Vesicular Transport Isn't Magic, It's Logistics
Most people think of vesicular export as this elegant cellular process and they're not wrong, but calling it elegant implies some forethought that doesn't actually exist. What's really happening is a series of mechanical sorting events, protein coat assembly, membrane curvature, and cargo selection that has been refined over billions of years through blunt evolutionary pressure rather than design. I spent four years studying this stuff in grad school and honestly the more I learned the less mystical it became.The Mysterious World Of Vesicular Export How Proteins And Lipids Are Packed And Transported
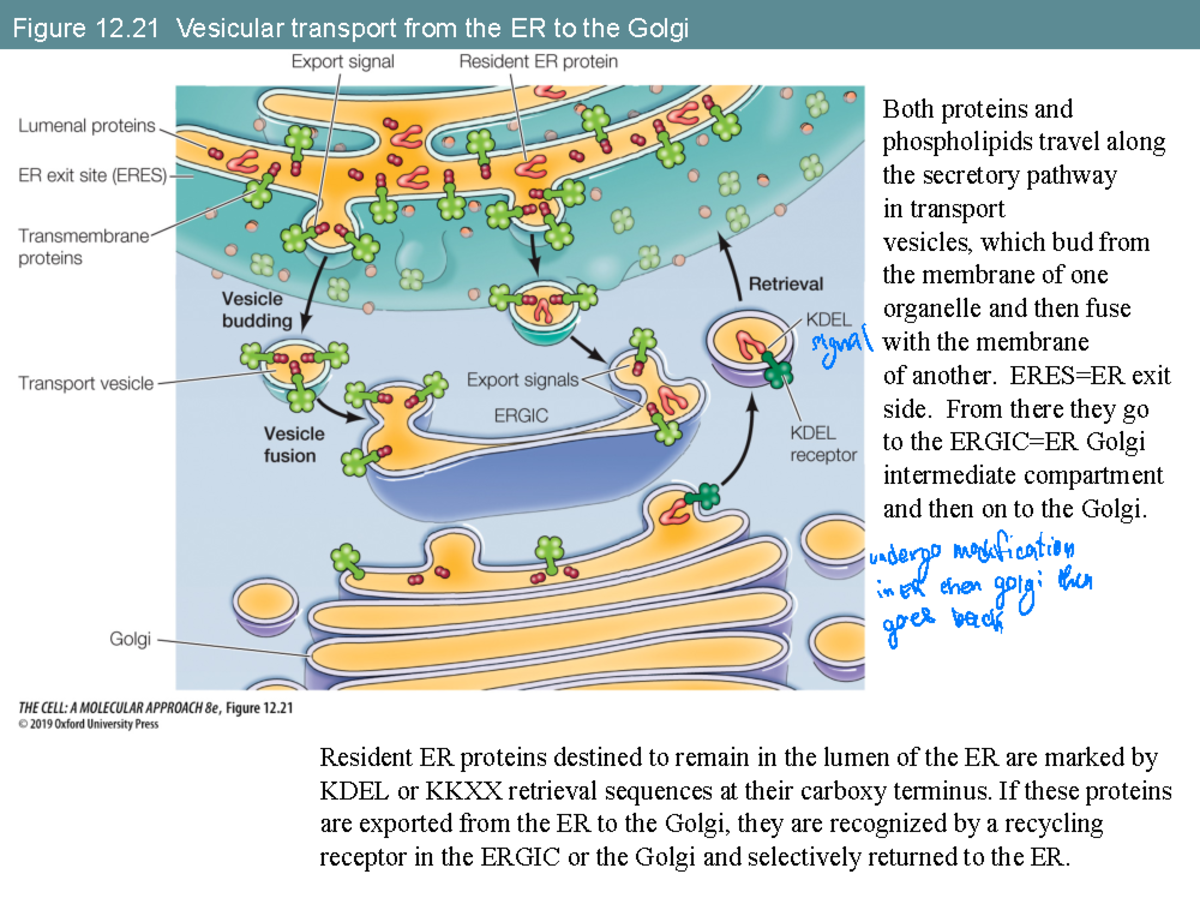
Vesicular export moves proteins and lipids from the endoplasmic reticulum through the Golgi apparatus and out to their final destinations. The basic machinery involves coat proteins like COPII for ER-to-Golgi transport, clathrin for later steps, and ADP-ribosylation factors that act as molecular switches. Cargo isn't just passively floating around waiting to be picked up. Specific signal sequences on transmembrane proteins and lipid head groups get recognized by adaptor complexes that cluster those molecules into budding vesicles. The ER exit sites are where this gets interesting. Not every part of the ER membrane participates in vesicle formation. You get concentrated zones where SEC16 proteins scaffold the assembly machinery and where cargo receptors like ERD2 for acidic hydrophilic tail fetch receptors collect their passengers. I remember running gel electrophoresis on fractions from a microsomal prep and seeing that certain glycosylated proteins were almost entirely absent from the secretory fraction until I realized I'd left the temperature on the water bath too high during the permeabilization step. The vesicles hadn't budded properly because the GTPase cycle had desynchronized. Fixed it by dropping the incubation to room temperature and adding excess Sec12 to drive guanine nucleotide exchange at the right rate. Lipid sorting works differently than protein sorting. Lipids don't carry signal peptides the way proteins do. They get selectively incorporated based on their physical properties and interactions with the coat. Ceramide, for instance, tends to partition into non-budding membrane regions while phosphatidylcholine concentrates in the curved necks of forming vesicles. This asymmetry matters because it means the lipid composition of the ER membrane is fundamentally different from the plasma membrane and every vesicle that shuttles between them carries that difference forward.
The Coat Assembly Problem
COPII coats assemble in a specific sequence that most textbooks oversimplify. Sar1-GTP inserts into the ER membrane, recruits Sec23/Sec24 heterodimers, which then bring in Sec13/Sec31 outer cage proteins. The whole process takes maybe thirty seconds under normal conditions. Get any component out of balance and you either don't get vesicles or you get oversized abnormal carriers that can't fuse properly with the Golgi. I once tried expressing a mutant Sec13 that lacked its C-terminal amphipathic helix and expected the coats to just fail to close properly. What actually happened was worse. The mutant coats assembled but created irregular tubular structures that traffic couldn't resolve. It looked like the cell was trying to export collagen through a straw designed for antibodies. The cargo jammed, the Golgi swelled, and I ended up with a culture that died in forty-eight hours. Lesson learned about testing coat mutants incrementally rather than going straight for the full knockout. Golgi retention is another thing people get wrong. You'd think proteins meant for the Golgi would just have a retention signal. They don't. Most Golgi residents are retained because they're too quickly retrieved back to the ER via COPI-coated retrograde vesicles. The equilibrium favors Golgi localization not because of a parking brake but because of constant recycling. Remove the retrieval pathway and those proteins leak through to the cell surface within an hour.
Lipid Transport Through Vesicular Carriers
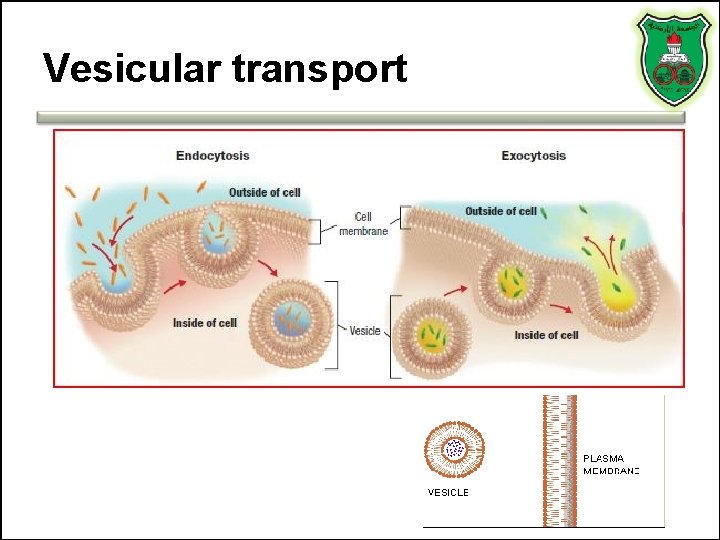
Lipid movement through vesicles is different from protein movement. Lipids flip-flop across bilayers slowly on their own, which is why flippases and scramblases exist. When a vesicle buds from the ER, the cytoplasmic leaflet gets packaged with the same lipid asymmetry as the source membrane. The luminal leaflet of the vesicle corresponds to the cytoplasmic leaflet of the target membrane after fusion. This matters for glycolipids and glycosylphosphatidylinositol-anchored proteins because their sugar modifications face the ER lumen during transport and end up on the extracellular side after the vesicle fuses with the plasma membrane. If you're doing lipid exchange experiments, be careful about using monocytes versus epithelial cells. Monocytes handle vesicular lipid transport very differently than polarized epithelial cells. I wasted two weeks trying to replicate a lipid raft partitioning study because the original paper used MDCK cells and I'd switched to HEK293 without realizing the transcytosis rates are completely different between the two. The lipid ratios looked wrong not because the mechanism was flawed but because the transport kinetics shifted the steady state.
Get the Full Details

Packing Efficiency and Cargo Capacity
Vesicles don't carry unlimited cargo. A typical COPII vesicle is about sixty to ninety nanometers in diameter and can hold roughly a thousand cargo molecules before the coat becomes unstable. This creates a real bottleneck when cells need to secrete large amounts of something like collagen or IgM antibodies. The cell solves this by forming larger carriers called mega-carriers or by clustering cargo receptors to increase packing density. There's also a problem with misfolded proteins clogging the export pathway. The ER has quality control mechanisms that retain misfolded proteins and target them for degradation through ERAD. But under stress conditions like ER calcium depletion or oxidative stress, the retention systems slow down and misfolded proteins can slip through into transport vesicles. This is why conditions like alpha-1 antitrypsin deficiency cause liver damage, not just lung damage. The misfolded protein accumulates in the ER of hepatocytes and eventually overwhelms the vesicular export system.
Practical Considerations for Working With This System
If you're studying vesicular export in a lab setting, your biggest enemy is probably temperature sensitivity. The entire process from coat assembly to vesicle fusion is tightly coupled to temperature through GTPase kinetics. A two-degree shift can change transport rates significantly. Always include temperature controls and check that your incubation conditions match the published protocols exactly. Drug inhibition is another minefield. Bafilomycin A1 inhibits the V-ATPase and indirectly affects vesicle maturation. Monensin disrupts Golgi pH and cargo sorting. Both are useful tools but they don't just stop vesicular export, they cascade into secondary effects that look like primary defects. If you see accumulation of a protein in the ER after monensin treatment, it could be because export is blocked or because the Golgi is so disrupted that retrograde signals aren't working properly. For quantitative work, consider using the sec mutant yeast system if you haven't already. The genetic tools available for studying vesicular transport in Saccharomyces cerevisiae are far more developed than in mammalian systems. The conservation is high enough that findings transfer well, and you can do pulse-chase experiments with radiolabeled amino acids that would be impossible in most mammalian cell lines. I switched from HeLa cells to yeast and cut my experimental timeline from months to weeks.
What This System Doesn't Do Well
Vesicular export is efficient but it's not perfect. The error rate in cargo selection is non-zero. Some proteins that shouldn't be secreted do get packaged, and some that should be retained don't make it through quality control. The system also can't handle rapid changes in demand very well. If a cell suddenly needs to secrete a flood of new proteins, the existing coat protein pool becomes limiting and there's a lag time before new synthesis catches up. There's also the problem of size constraints. Vesicular transport simply cannot move large structures like organelles or big protein complexes efficiently. For those, cells use other mechanisms like tunneling nanotubes or direct membrane continuity. Don't try to force everything through the vesicular pathway just because it's the most studied one.