How Trophic Levels Actually Work In Real Fieldwork
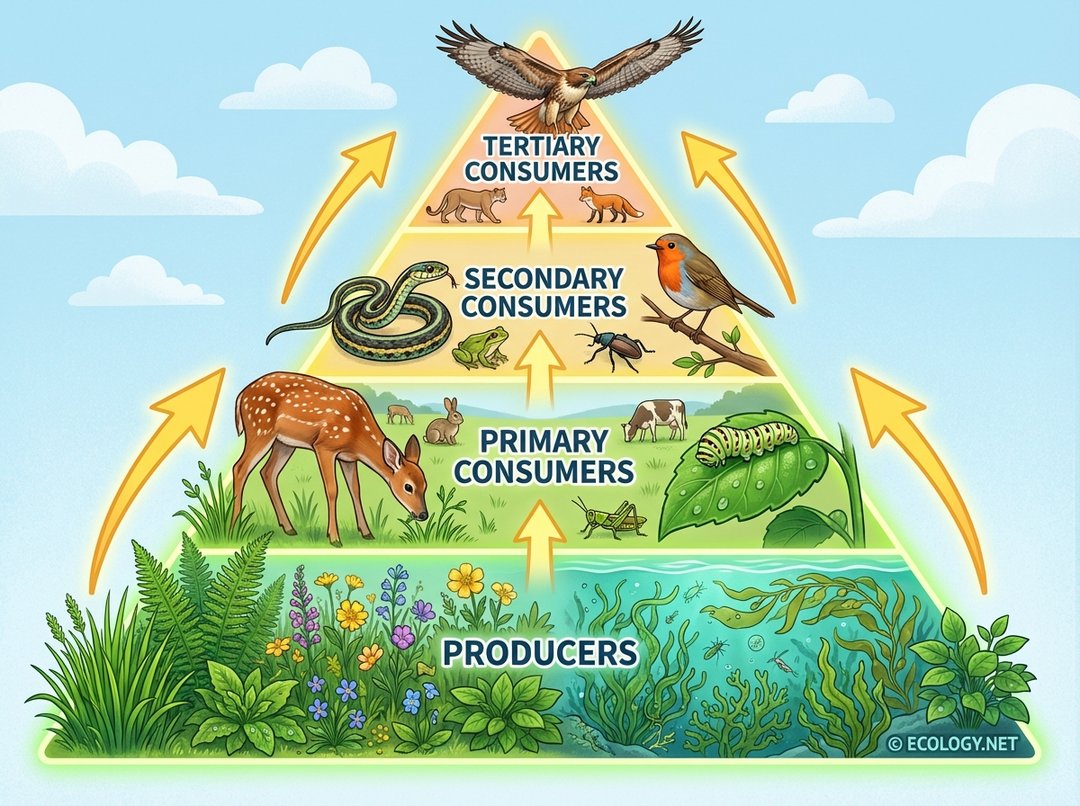
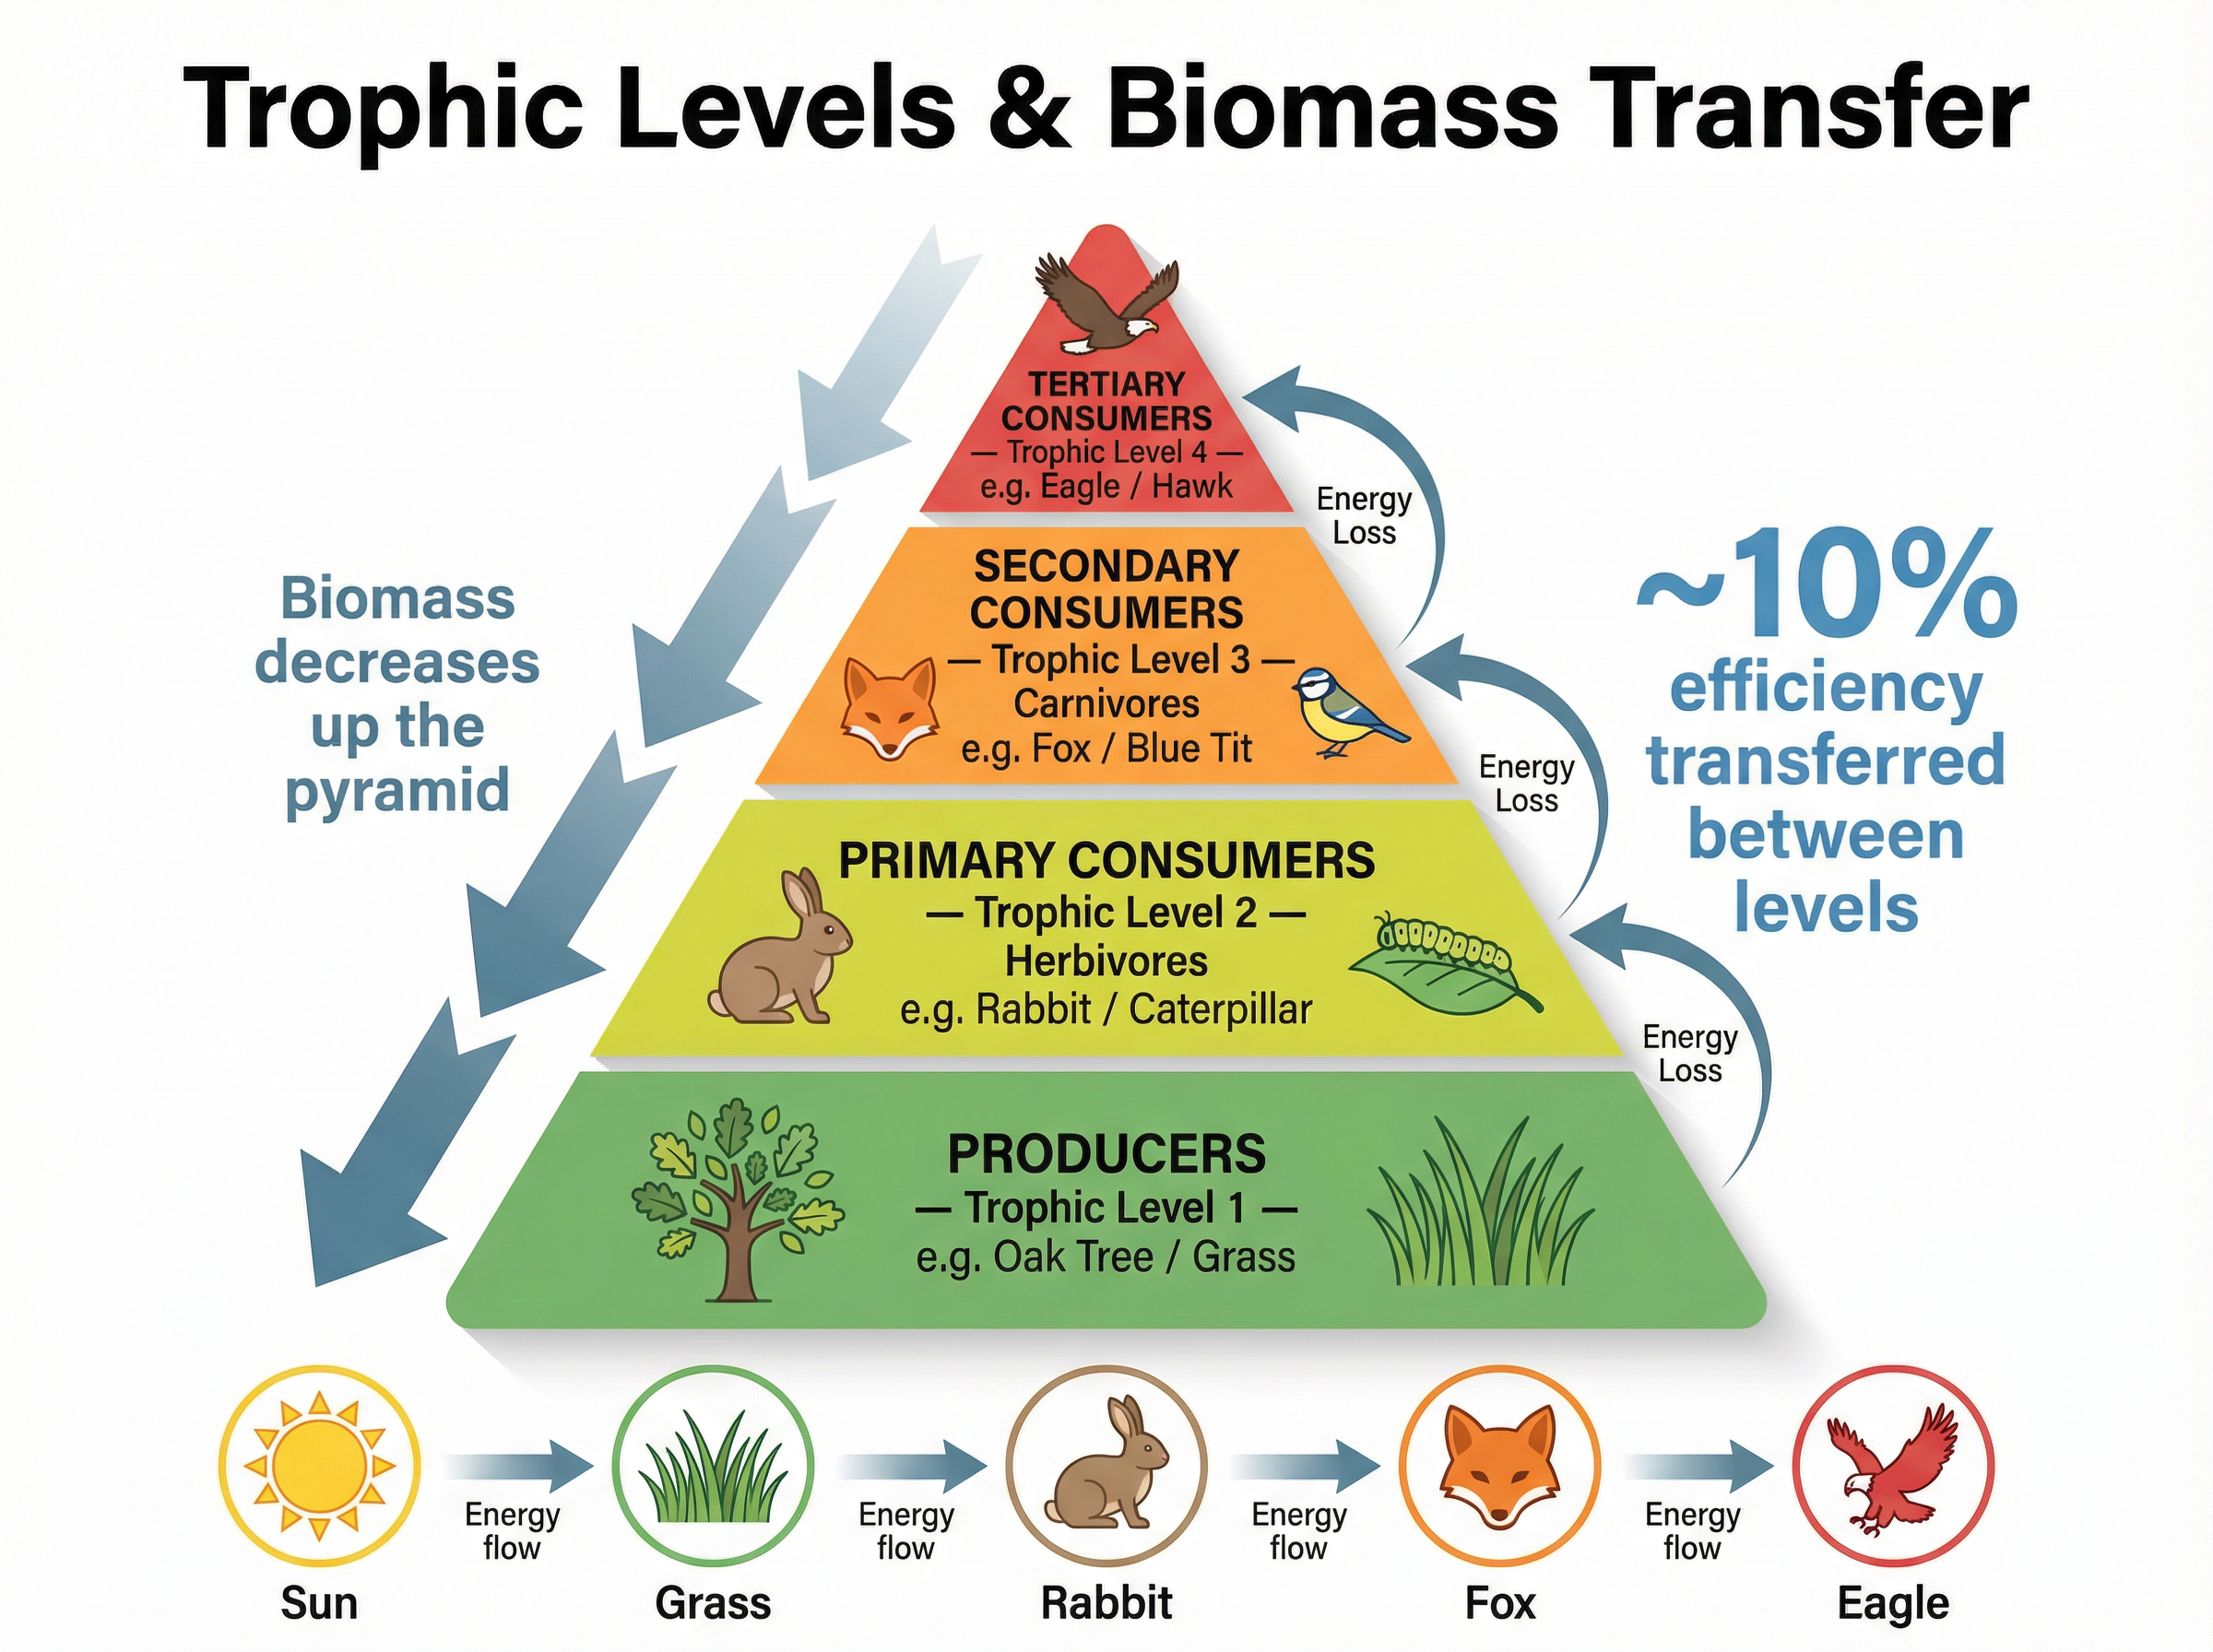
Most ecology textbooks present trophic levels as clean little rungs on a ladder. Producers sit at the bottom, herbivores climb up one step, carnivores go another, and decomposers get their own quiet corner at the end. In practice, ecosystems don't care about that neatness. I spent roughly six years sampling riparian food webs along the River Tay catchment, and the first thing you learn is that almost nothing fits cleanly into a single level. The concept itself is useful, sure, but treating it as a rigid hierarchy is how you end up with a dataset that makes zero sense when you try to model it. The basic mechanism is straightforward enough: energy enters an ecosystem through photosynthesis, moves through consumers, and degrades at each transfer. The 10 percent rule—roughly speaking, only about ten percent of energy at one level makes it to the next—is a starting point, not a law. In my work, I've seen transfer efficiencies swing from 3 percent in cold, nutrient-poor streams to over 20 percent in eutrophic estuaries. The variation matters because it determines how many levels an ecosystem can actually support before energy runs out.
The Hidden World Of Trophic Levels Unlocking The Secrets Of Ecosystems
Here's what most introductory material leaves out: the real structure of a food web isn't a pyramid, it's a mesh. Omnivory is the rule, not the exception. A brown trout in a Scottish burn will eat mayfly nymphs (primary consumer), yes, but it'll also take terrestrial insects that fall onto the water surface, and occasionally it'll eat its own young. That means the trout is simultaneously occupying two trophic levels depending on what it's eating that week. When I first tried to assign a single trophic level value to species in my early papers, my supervisor made me re-do the analysis after I pointed out that my model predicted negative biomasses for certain predator groups. The fix was using a continuous trophic level approach instead of discrete categories, which is standard practice now but wasn't when I started. The deeper insight people miss is that trophic level isn't just about who eats whom—it's about how energy flows through time. Seasonal pulses matter enormously. In temperate zones, the spring algal bloom supports a burst of primary production that cascades up the web. Zooplankton densities spike, fish larvae grow faster, and predatory insects follow. By autumn, the whole system compresses. If you sample once in May and once in October and assume the trophic structure is the same, your conclusions will be wrong. I learned this the hard way after submitting a paper that claimed a stream had a stable four-level food chain when in reality it oscillated between three and five levels depending on the season. Stable isotope analysis has changed how we measure this stuff. Instead of watching what organisms eat in the wild—which is tedious and often inaccurate—you measure the ratios of nitrogen-15 to nitrogen-14 in tissue. Each step up the food web enriches the sample by roughly 3 to 4 per mil. That gives you a direct read on an organism's integrated trophic position over weeks or months, depending on turnover rate. The caveat is that baseline isotopic signatures vary spatially. Two streams fifty kilometers apart can have completely different starting isotope values, so you can't just apply a universal enrichment factor. I've seen people cite trophic levels from published literature without measuring local baselines, and the resulting errors were substantial—sometimes shifting a species' inferred trophic position by over half a level.
Another counter-intuitive point: higher trophic levels aren't always the top predators. In many aquatic systems, the so-called "top predator" is itself heavily preyed upon by migrating birds or larger fish that move through seasonally. The Arctic char in lochs like Loch Lomond might sit at trophic level 4.2 during summer, but when vendace move in during autumn, the char's effective trophic level drops because it becomes prey. This vertical mobility of trophic position is something traditional models completely ignore, and it's why some ecosystems appear less stable than they actually are when you look at them through a static lens. There's also the detrital pathway that textbooks bury in a footnote. A huge amount of energy in most ecosystems flows through dead organic matter rather than living producers. In forest streams, leaf litter can be the dominant energy source, and the organisms that process it—caddisfly larvae, stonefly nymphs, shredding amphipods—sit at trophic level 2 even though they're consuming dead plant material, not living plants. This splits the system into two parallel food webs: the grazing web and the detrital web. They're connected, but they operate on different timescales and respond differently to disturbance. When I logged canopy removal along a tributary, the grazing web collapsed within weeks while the detrital web actually increased initially because more light meant more algal growth on the remaining leaves. The net effect on fish biomass took two years to resolve, and in the interim my trophic level calculations based on a single-web model were misleading. If you're building your own analysis, start by deciding whether discrete or continuous trophic levels fit your question. For community-level patterns, continuous values from isotope data are far more informative. For classroom explanations or broad comparative studies, discrete levels are acceptable if you acknowledge the simplification. Don't try to force every organism into a box. The systems that work best in practice are the ones that leave room for the messy middle—those generalist feeders and opportunistic predators that hold the whole structure together.
Get the Full Details

The main limitation of the trophic level framework is that it reduces a multidimensional reality to a single number. Two species can share the same trophic level but occupy completely different niches—one might be a benthic insectivore and the other a pelagic planktivore, for example. If your management decision depends on understanding competitive dynamics or energy pathway specificity, trophic level alone won't cut it. In those cases, network analysis or mixing models give you more resolution, though they require more data and more effort to interpret correctly. I still use trophic levels in my work because they're useful shorthand, but I've stopped pretending they capture the full picture. The secret isn't in the levels themselves—it's in understanding what the gaps between them represent, and how energy actually moves through those gaps under real-world conditions.