What Meiosis Actually Does When You're Not Paying Attention
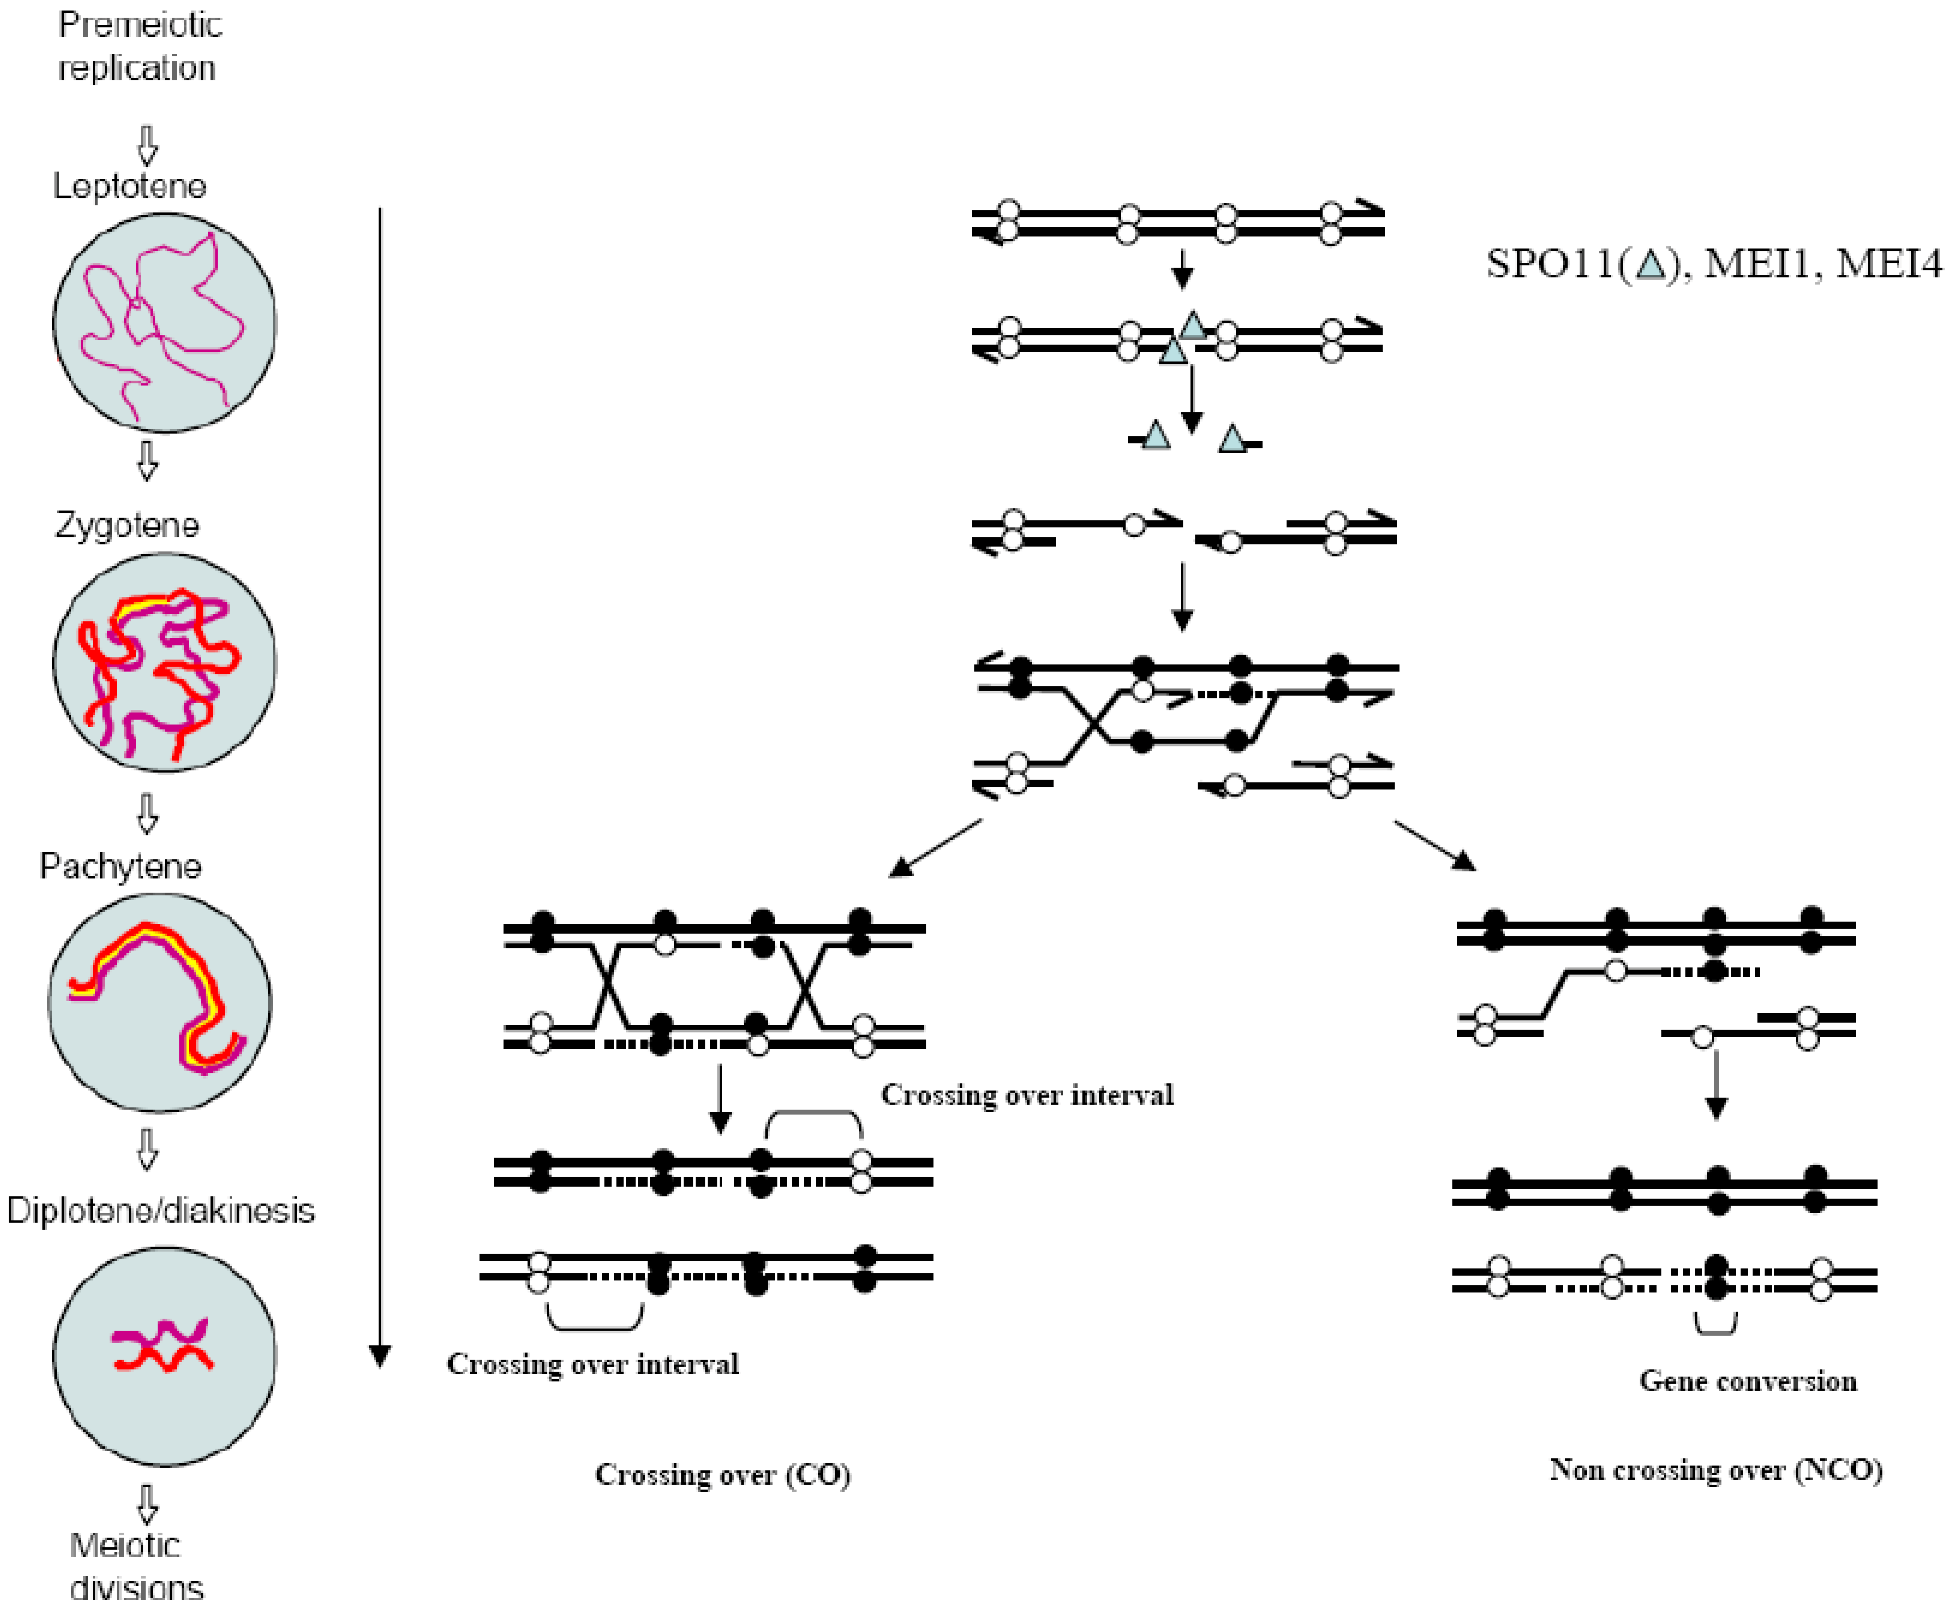
Most people think meiosis is just the textbook diagram with chromosomes lining up and splitting. It is that, but the interesting part is what happens between the lines. The recombination step during prophase I is where the actual work happens, and it is not as clean as you were taught. When homologous chromosomes pair up during zygotene, they form something called a synaptonemal complex. This is a protein scaffold that holds the two chromosomes in tight alignment. Then in pachytene, crossovers happen. DNA strands break and rejoin across the homologs. This is crossing over. It shuffles alleles between maternal and paternal chromosomes. The result is recombinant chromatids that are neither purely maternal nor purely paternal. That reshuffling is the engine of genetic diversity in sexually reproducing organisms.The Hidden Superpowers Of Meiosis How Cellular Recombination Fuels Evolution And Survival
Here is what most people miss about recombination. It is not random in the way beginners assume. Recombination hotspots exist. In humans, the PRDM9 protein determines where crossovers happen by binding specific DNA sequences. Some species have hotspot locations that shift rapidly over evolutionary time because PRDM9 itself evolves. This means the very places where recombination occurs are in constant flux. That is a problem for genome assembly and for understanding disease mapping. I spent months trying to reconcile linkage data from a set of plant genomes where the expected recombination map did not match any published reference. The issue turned out to be a recently inserted transposon near a hotspot that was suppressing crossover activity in that region. The workaround was to use a different population with higher historical recombination rates in that locus and build a pedigree-based map instead of relying on the reference. It added about three weeks of sequencing and analysis but saved the project.
How Recombination Actually Drives Evolution
Recombination breaks up linkage between alleles. That sounds abstract until you think about what it means for selection. Without recombination, a beneficial mutation has to wait for a back mutation or a separate event to escape a bad genetic background. This is Muller's Ratchet. In asexual populations, deleterious mutations accumulate irreversibly. Recombination lets beneficial alleles combine onto the same chromosome and lets selection purge bad combinations independently. Another thing that does not get enough attention is the role of recombination in creating novel allele combinations that selection can act on. Most of the time, the individual crossovers produce variations that are neutral or slightly deleterious. But occasionally, a new combination confers something useful. The 2016 study on stickleback fish showed that repeated recombination events at specific loci allowed freshwater populations to independently evolve similar armor plate reductions. The same genetic solutions kept appearing because recombination was generating them at predictable frequencies.
Technical Details Most Beginners Skip
Meiosis has two divisions. Meiosis I separates homologous chromosomes. Meiosis II separates sister chromatids. The recombination event happens before either division, during prophase I. The physical crossover is visible as a chiasmata, the X-shaped structure holding homologs together until anaphase I. Without at least one chiasmata per chromosome pair, the spindle cannot orient the bivalent correctly and nondisjunction becomes likely. That is why there is a minimum crossover requirement. There is also crossover interference. When one crossover forms, the chance of another forming nearby drops significantly. The mechanism is not fully resolved but it involves mechanical stress along the synaptonemal complex and signaling through the ATM kinase pathway. This means crossovers are spread out rather than clustered, which actually helps ensure proper segregation.
Get the Full Details

Where The System Fails
Recombination is not universally beneficial. There are scenarios where it causes real damage. Chromosomal rearrangements like translocations and inversions can suppress recombination in heterozygous individuals because the misaligned chromosomes produce unbalanced gametes. This is a major reason why some species have large inverted regions that stay frozen as co-adapted gene complexes. The classic example is the supergene controlling mating morphs in the ruff bird. Recombination within the inversion would break apart the favorable combination of alleles, so selection maintains the suppression. Another failure mode is non-allelic homologous recombination. When sequence similarity exists between non-homologous regions, crossover can happen at the wrong place. This causes copy number variations and is a known mechanism behind several genetic disorders. Williams syndrome, for example, results from a recurrent deletion caused by recombination between low-copy repeat sequences. This is not a rare edge case. It happens frequently enough that clinical geneticists screen for these hotspot-prone regions.
What This Means In Practice
If you are working with genetic data and trying to understand recombination patterns, do not assume uniform crossover distribution. Use high-density SNP maps or direct cytological staining of MLH1 foci to see where crossovers actually occur in your system. MLH1 marks the sites of crossover resolution and gives you a direct readout of recombination events per cell. This approach typically takes about two days from sample prep to counting, but it is far more accurate than inferring recombination rates from linkage alone. The downside of relying on recombination as an evolutionary engine is that it requires sex. And sex is costly. It takes twice as long to produce offspring compared to asexual reproduction, and you only pass on half your genome. The fact that most complex life still uses sex despite these costs is one of the strongest arguments for how important meiotic recombination actually is. Without it, adaptation slows down dramatically and mutation load becomes unsustainable over long timescales. The machinery behind all of this is conserved from yeast to humans. The core proteins involved in strand invasion, Holliday junction formation, and resolution are largely the same. RAD51 and DMC1 handle the homology search. MUS81 and GEN1 resolve the junctions. If any of these are mutated, recombination efficiency drops and meiotic errors increase. In humans, mutations in these genes are associated with infertility and increased risk of aneuploidy in offspring.