Osmosis and Diffusion in Practice
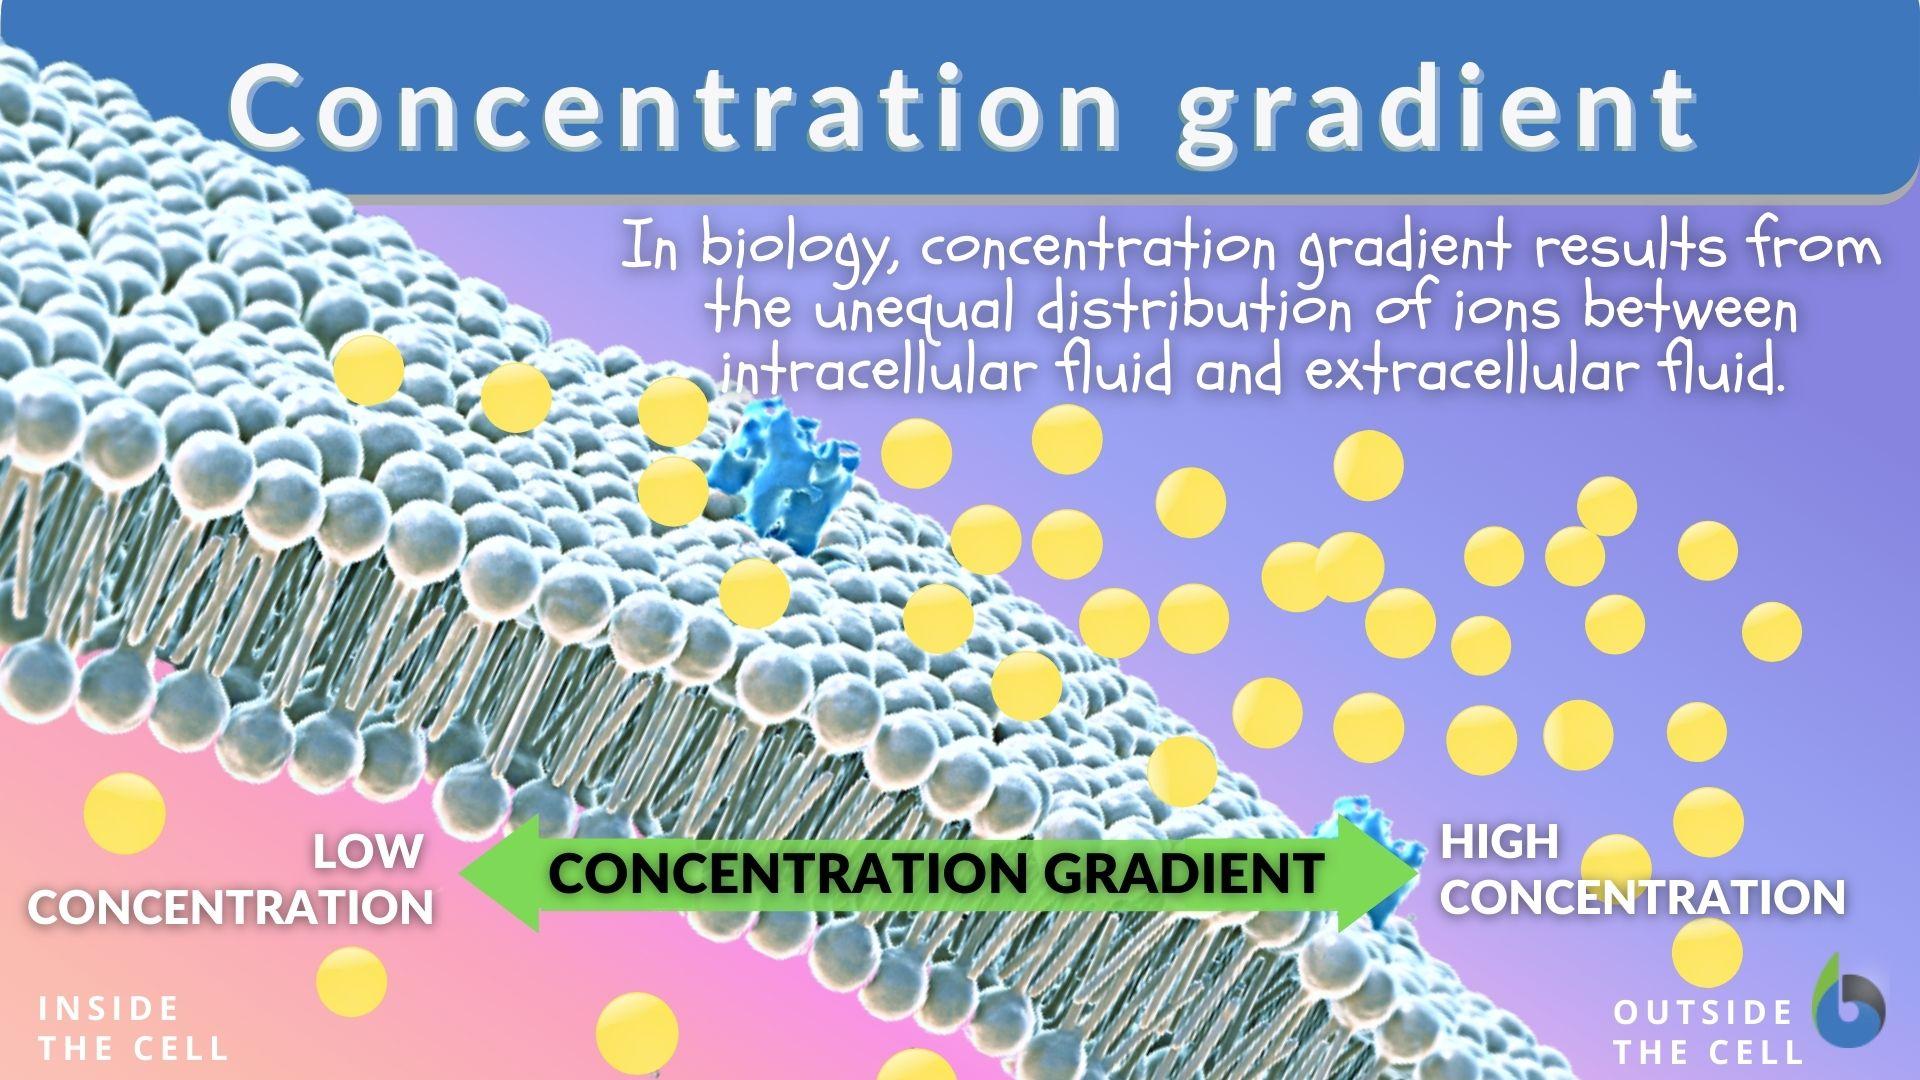
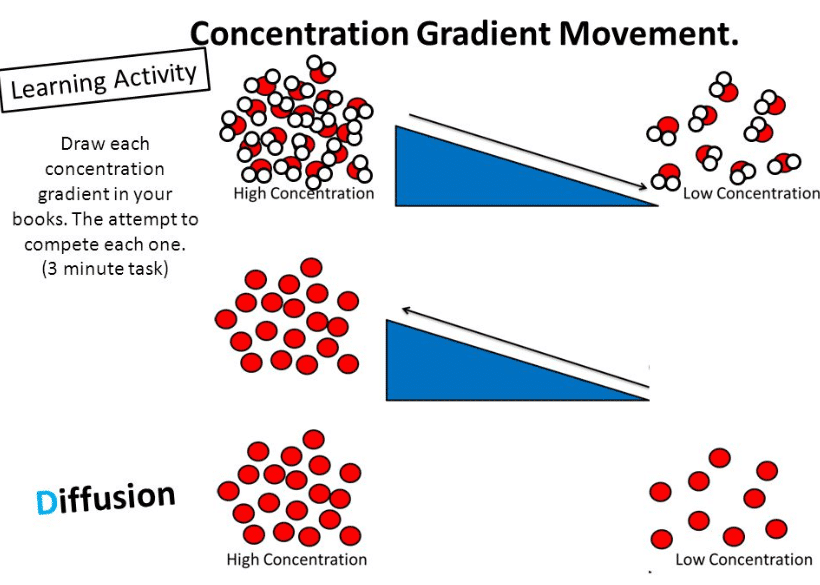
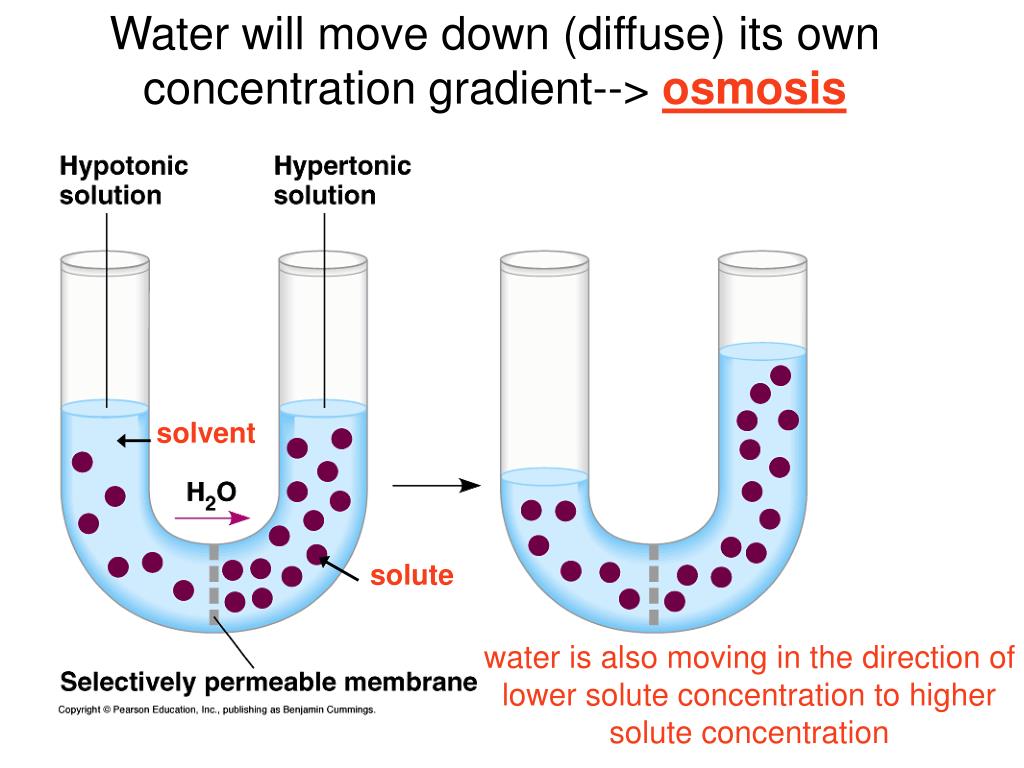
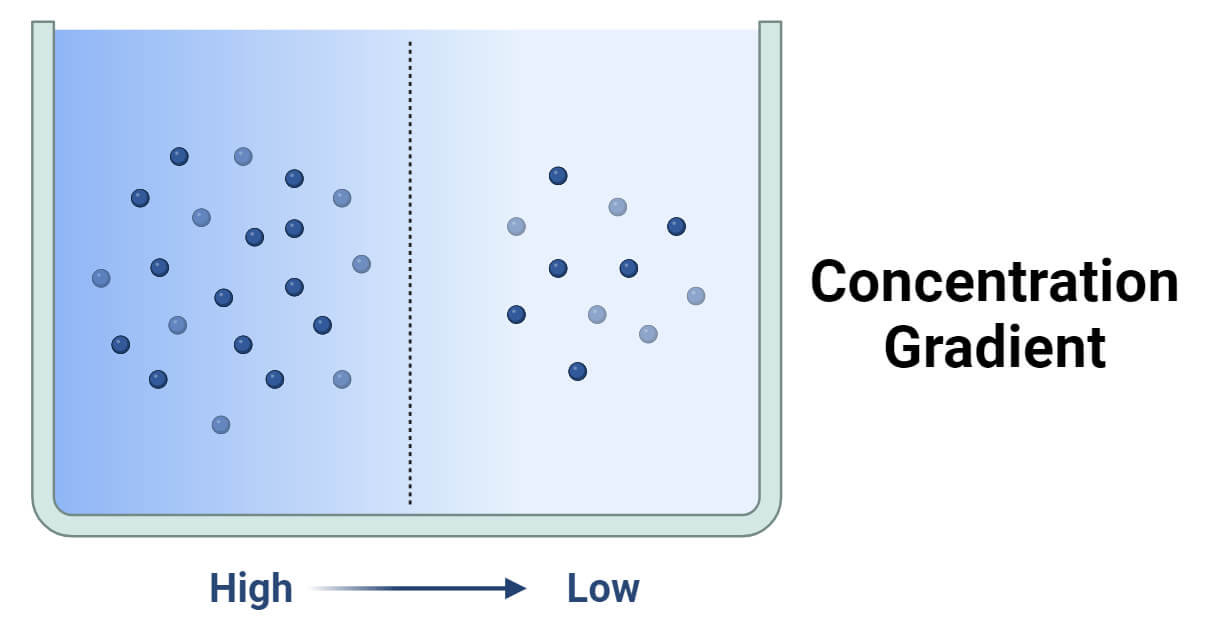
When you set up a dialysis experiment in the lab, the first thing you notice is that nothing dramatic happens for a while. The solution in the bag looks identical to the beaker around it. Then, over hours or sometimes days, the concentration equalizes. This is the physical reality behind When Molecules Move Down Their Concentration Gradient A Fundamental Concept In Chemistry. It is not instantaneous, and it is not always smooth. A concentration gradient exists whenever there is a difference in solute concentration between two regions. Molecules will naturally move from the area of higher concentration toward the area of lower concentration until equilibrium is reached. This is driven by the random thermal motion of particles, not by any conscious direction. The process requires no external energy input, which is why it is classified as passive transport. In a laboratory setting, this principle shows up repeatedly. I once ran a permeability assay using a cellulose membrane with a 12,000 Dalton molecular weight cutoff. I loaded a solution of glucose on one side and pure water on the other. The expected result was a measurable shift in osmotic pressure as water moved across the membrane. Instead, the readings were inconsistent because the membrane had dried out during storage and the polymer chains had collapsed, narrowing the effective pore size. I had to rehydrate the membrane for six hours in isotonic saline before the data became reliable. That is the kind of detail textbooks do not emphasize but practical work demands.
The mathematical description relies on Fick's laws of diffusion. The first law states that the flux of particles is proportional to the concentration gradient, expressed as J = -D(dC/dx), where D is the diffusion coefficient and dC/dx is the change in concentration over distance. The negative sign indicates movement from high to low concentration. The second law describes how concentration changes over time in a non-steady-state system, which is more relevant to real experiments where the gradient itself shifts as diffusion proceeds. Several factors influence the rate at which this movement occurs. Temperature is a primary variable because kinetic energy increases with heat, causing molecules to move faster and collide more frequently. Molecular size matters significantly. A small ion like potassium crosses a membrane orders of magnitude faster than a protein, even through the same pathway. The medium also plays a role. Diffusion in water is roughly ten thousand times faster than in a viscous cytoplasm, which is why intracellular transport relies heavily on motor proteins rather than waiting for passive movement. Membrane permeability introduces another layer of complexity. A phospholipid bilayer is selectively permeable, allowing small nonpolar molecules like oxygen and carbon dioxide to pass freely while blocking charged species and large polar molecules. When considering biological systems, this selectivity means that not all concentration gradients dissipate at the same rate. Ion channels and transporters create controlled pathways that can accelerate or restrict movement beyond what simple diffusion would predict.
I encountered a particularly stubborn case involving ethidium bromide staining of agarose gels. The dye needed to migrate into the gel and bind DNA, but the standard soaking protocol took overnight. I found that increasing the temperature to 37 degrees Celsius and adding a brief vacuum infiltration step cut the staining time to under thirty minutes without compromising resolution. The key was understanding that raising temperature increased the diffusion coefficient while the vacuum temporarily disrupted the concentration boundary layer at the gel surface, allowing fresh dye to contact the gel matrix more rapidly. One counter-intuitive point that beginners often miss is that equilibrium does not mean all movement stops. At equilibrium, molecules continue to move randomly in both directions, but the net flux is zero because the rates are equal. This dynamic equilibrium is important when interpreting experimental results. A measured concentration of zero on one side of a membrane does not necessarily mean nothing is crossing—it could mean the system has reached equilibrium and the forward and reverse rates balance each other. Another common misunderstanding involves the assumption that smaller gradients always lead to proportionally slower diffusion. While Fick's law does show a linear relationship between flux and gradient magnitude, real systems often deviate from this ideal. In crowded cellular environments, molecular crowding can cause anomalous diffusion where the mean squared displacement does not scale linearly with time. This makes predictions based purely on dilute solution mathematics unreliable in biological contexts.
Get the Full Details

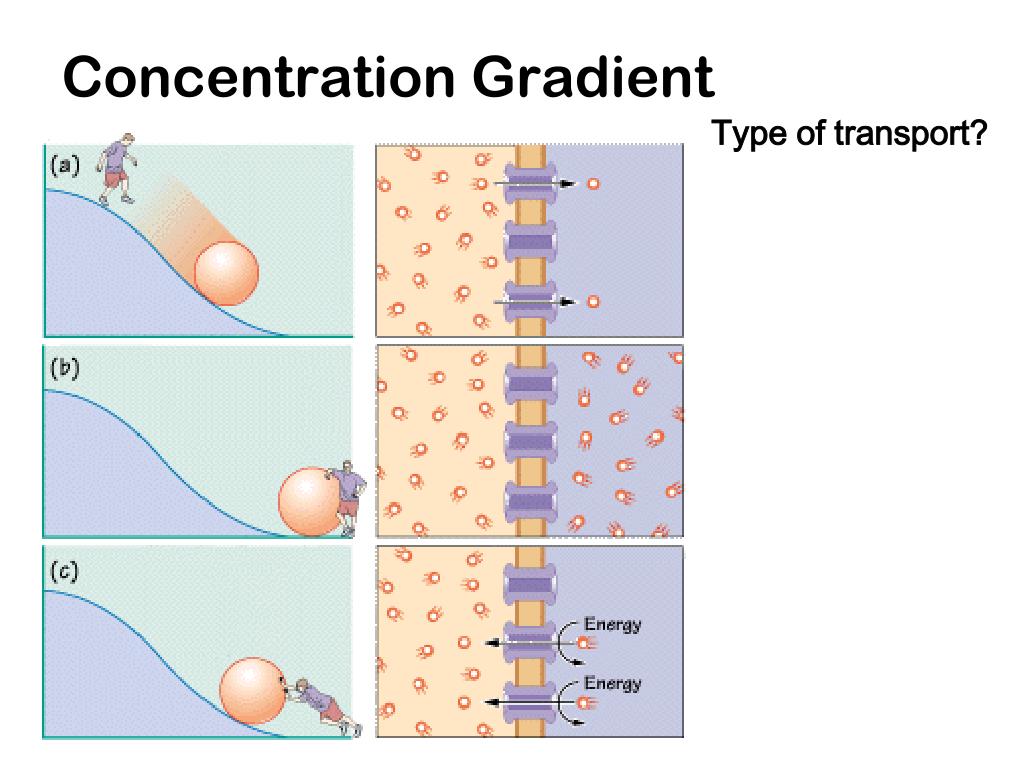
There are scenarios where this concept fails to provide useful predictions. In systems with active transport mechanisms, molecules move against their concentration gradient using energy from ATP hydrolysis. The sodium-potassium pump is a classic example, maintaining a steep electrochemical gradient that would spontaneously collapse if left to passive processes alone. Attempting to model such systems with Fick's laws will produce incorrect results because the underlying assumption of passive movement is violated. Similarly, in porous media with complex geometry such as soil or biological tissue, the effective diffusion coefficient can differ substantially from the value measured in free solution. Tortuosity, defined as the ratio of the actual path length a molecule must travel to the straight-line distance, reduces the effective rate of transport. In brain tissue, for instance, extracellular diffusion is approximately four times slower than in water due to the obstructed pathways created by cells and extracellular matrix components. For practical applications, whether you are designing a drug delivery system or interpreting physiological data, the critical variables to track are temperature, molecular weight, membrane properties, and the presence of any carrier proteins or channels. If you are working with synthetic membranes, always verify the hydration state and store them according to manufacturer specifications. Dried membranes behave differently from hydrated ones, and the difference is not always reversible.
The concept itself is straightforward, but applying it correctly requires attention to the conditions under which it operates. Passive movement down a concentration gradient is a foundational mechanism, but it is one among several that govern molecular transport in real systems. Understanding its limits is as important as understanding its operation.