Protein Synthesis Is More Messy Than Textbooks Admit
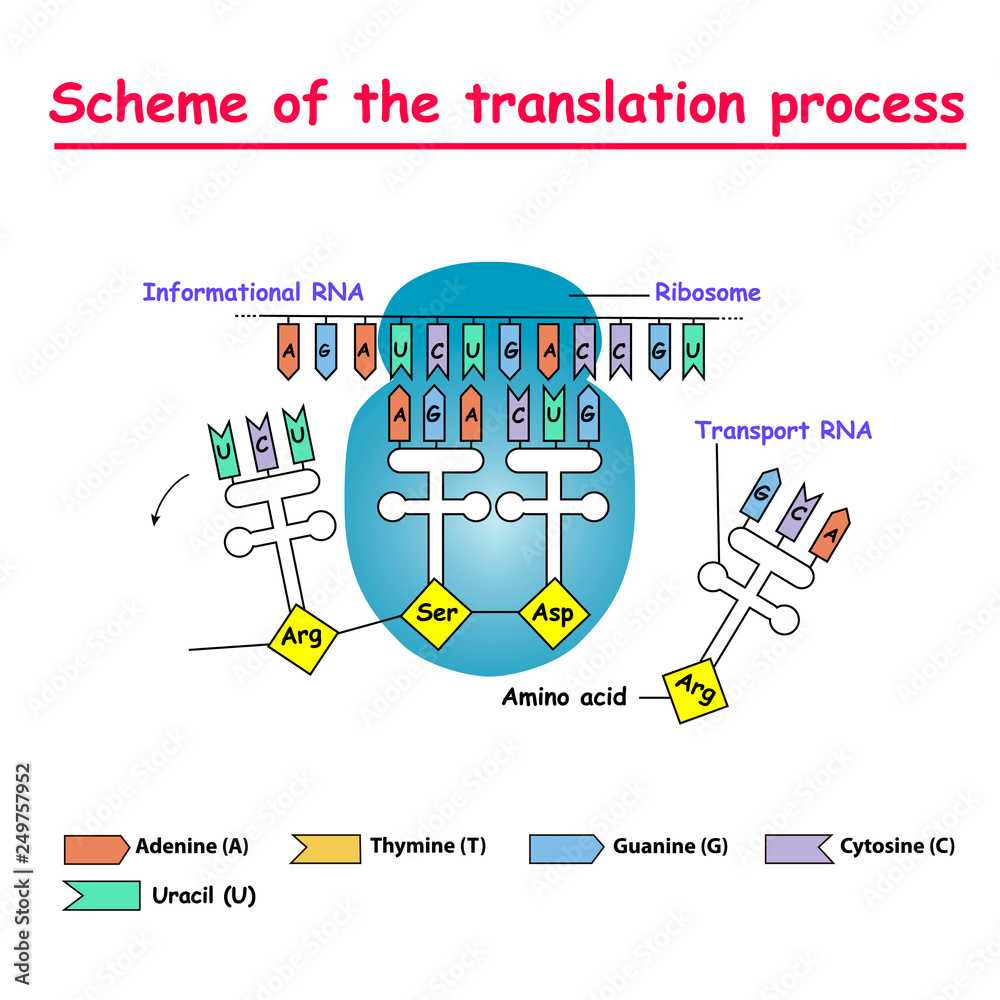
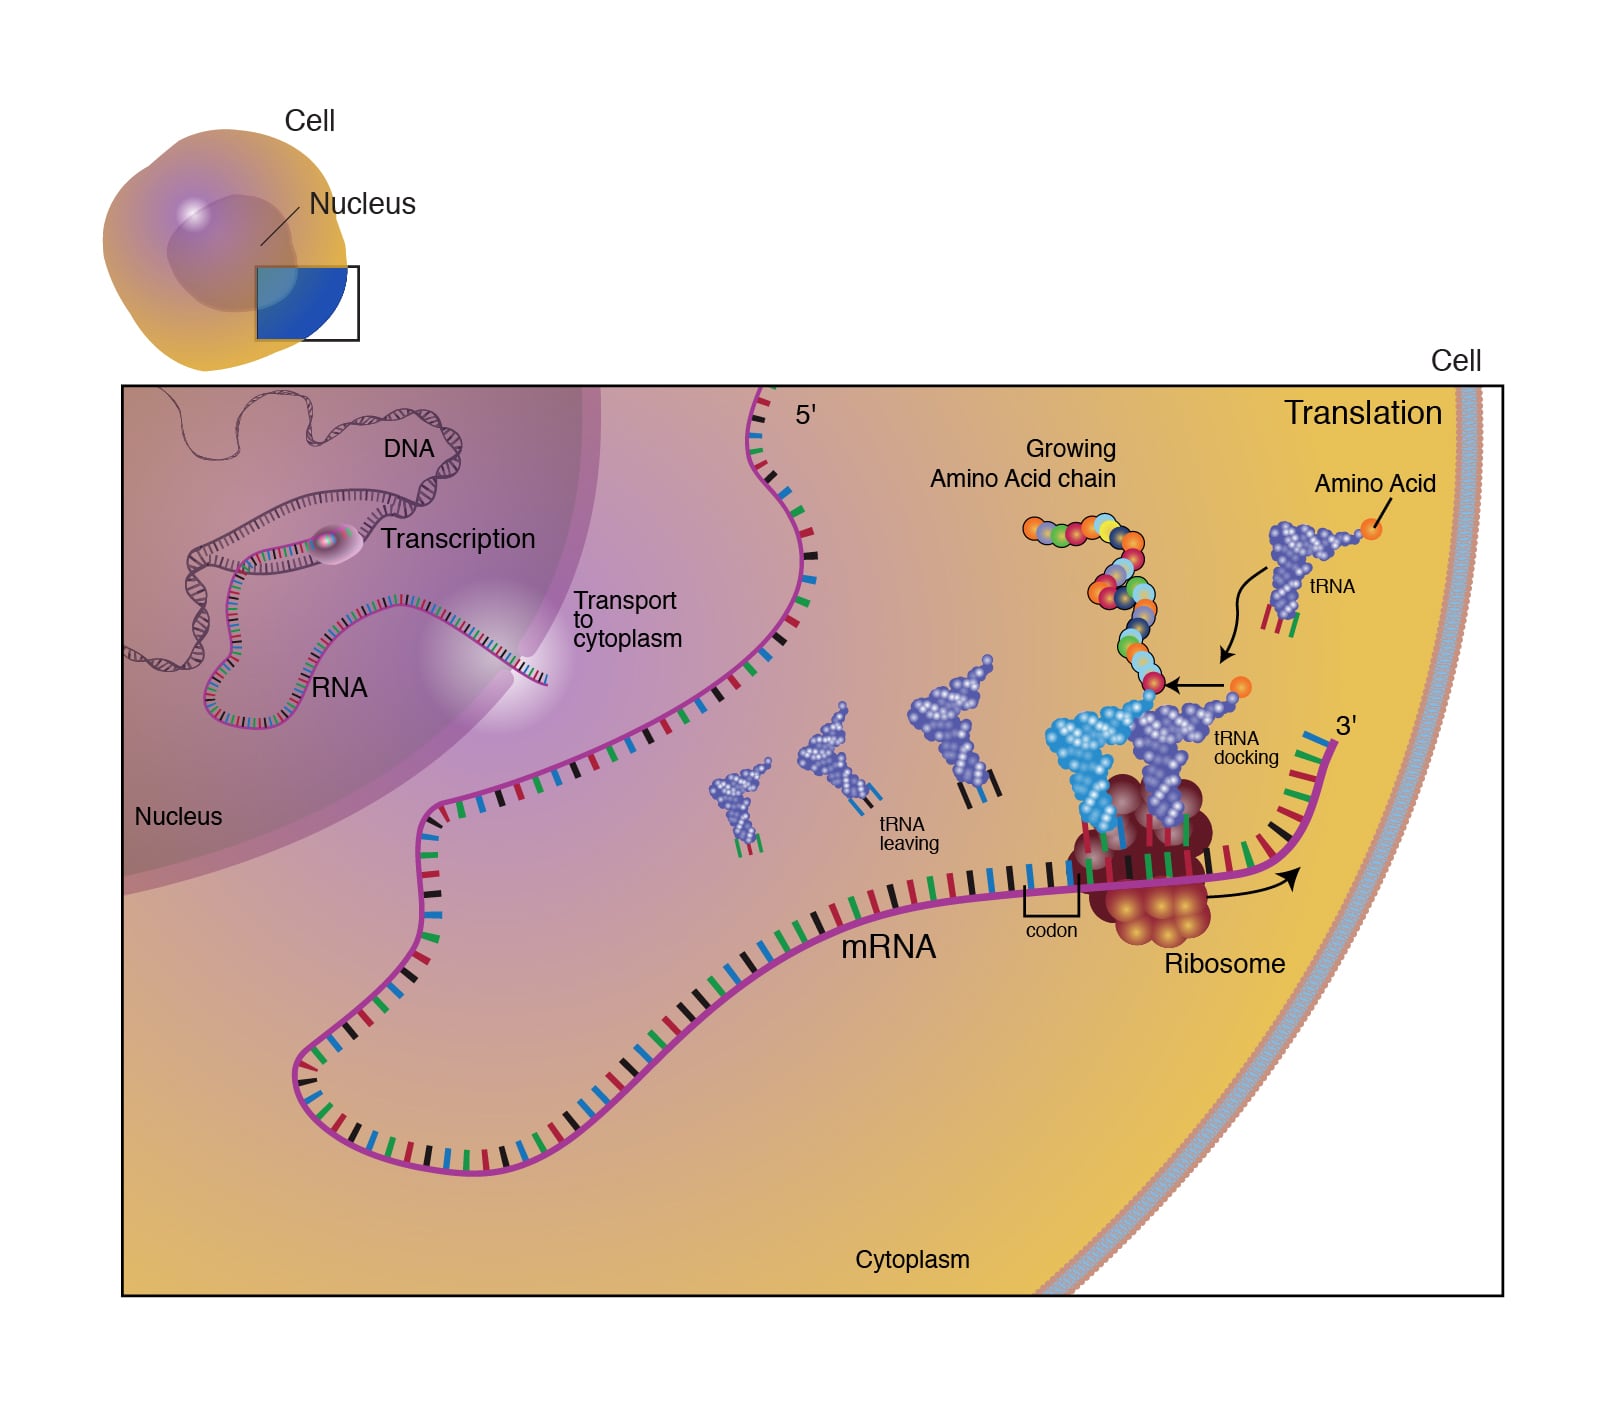
Translation is the process where ribosomes read messenger RNA and assemble amino acids into polypeptide chains. That is the textbook answer. The reality involves a lot of regulatory checkpoints, quality control failures, and edge cases that standard biology courses barely scratch the surface of. The core mechanism is straightforward enough. You have mRNA coming off the DNA, a ribosome that acts as the physical machinery, transfer RNAs carrying specific amino acids, and a whole cast of protein factors that help everything run in the right order. Initiation, elongation, termination. That is the basic arc. But the interesting stuff happens in the details.
What Is Translation In Biology Decoding The Molecular Mechanism That Builds Life
The genetic code is degenerate, which means multiple codons can specify the same amino acid. This was one of those things I learned years into working with expression systems before it actually made sense to me. It is not just a curious footnote. It has real consequences for how you design constructs and interpret results. I spent about three weeks troubleshooting a recombinant protein that refused to express in E. coli at the expected yield. The gene sequence was correct, the promoter was fine, the induction conditions were standard. The problem turned out to be codon bias. The mRNA had a stretch of rare arginine codons that the bacterial translation machinery simply could not process efficiently. The ribosome would stall, and the whole system would degrade the transcript through quality control pathways. Switching to a codon-optimized version of the gene and using a strain with extra tRNA supplements solved it. Expression went from nearly undetectable to roughly 15 milligrams per liter of culture. That is the kind of practical detail you do not pick up from a general overview.
Initiation Sets the Pace for Everything Else
In eukaryotes, the 40S ribosomal subunit binds to the 5' cap of the mRNA along with initiation factors, then scans downstream until it finds an AUG start codon in the right context. The Kozak sequence matters here. A strong Kozak consensus surrounding the start codon can dramatically improve translation efficiency. A weak one often results in leaky scanning, where the ribosome bypasses the first AUG and initiates further downstream, producing a truncated or entirely different protein. In prokaryotes, the mechanism is different. The Shine-Dalgarno sequence upstream of the start codon base-pairs with the 16S rRNA of the 30S subunit, positioning the ribosome directly at the initiation site. No scanning required. This is why putting a prokaryotic ribosome binding site upstream of your gene is essential if you are working in bacterial systems. Without it, translation initiation is essentially random and usually very inefficient. One counter-intuitive thing about initiation is that it is often the rate-limiting step, not elongation. People tend to focus on codon optimization for speed, but the real bottleneck is usually getting the ribosome loaded onto the mRNA in the first place. Strong initiation signals paired with moderate elongation rates often outperform weak initiation with maximally optimized codons.
Get the Full Details

Elongation Is Where Things Actually Go Wrong
During elongation, aminoacyl-tRNAs deliver their cargo to the ribosome's A site. The correct tRNA is selected through codon-anticodon pairing, GTP is hydrolyzed by elongation factor eEF1A in eukaryotes or EF-Tu in prokaryotes, and the growing chain is transferred to the new amino acid via peptidyl transferase activity in the large ribosomal subunit. Then translocation moves the ribosome forward by one codon. The fidelity of this process is remarkably high, around 10^-4 to 10^-5 per codon. That means roughly one mistake for every 10,000 to 100,000 amino acids incorporated. For most proteins that is fine. For long proteins or proteins with specific structural requirements, even low error rates become significant over time. Misfolded proteins accumulate, and cellular quality control mechanisms like chaperones and the ubiquitin-proteasome system have to deal with the fallout. I ran into a case where a apparently silent mutation in a viral gene reduced protein expression by about 40 percent. The mutation did not change any amino acids, but it created a stable secondary structure in the mRNA that caused the ribosome to pause. Those pauses disrupted co-translational folding. The protein that did get made was misfolded and targeted for degradation. This is one of those things that is easy to overlook because the sequence looks identical at the protein level. You have to actually predict mRNA structure or test it empirically to catch it.
Ribosome stalling can also be triggered by rare codons, but it is not just about tRNA availability. Structural elements in the mRNA, modified bases in tRNAs, and even the amino acid sequence of the growing peptide chain itself can all cause translational pauses. These pauses are not always a problem. In some cases they are functionally important, giving domains time to fold correctly before the next one is synthesized. The ribosome is not a dumb assembly line. It coordinates with folding chaperones and other cellular machinery in real time.
Termination and What Comes After
When a stop codon enters the A site, release factors recognize it and catalyze the hydrolysis of the peptidyl-tRNA bond, releasing the completed polypeptide. In eukaryotes, eRF1 does this work. In prokaryotes, RF1 and RF2 handle the three stop codons in a redundant fashion. After release, the ribosome dissociates into its subunits, ready to be recycled. But the story does not end there. The newly synthesized polypeptide typically needs post-translational modifications to become functional. Glycosylation, phosphorylation, disulfide bond formation, proteolytic cleavage. These happen in the endoplasmic reticulum and Golgi apparatus in eukaryotes, or in the periplasm and cytoplasm in prokaryotes. Getting the translation mechanism right is only the first step. If your expression system cannot perform the necessary modifications, you will have a perfectly translated protein that is biologically inactive. This is especially relevant when you are expressing eukaryotic proteins in bacterial systems. Bacteria lack the organelles for complex post-translational modifications. They also do not have the same redox environment for disulfide bond formation in the cytoplasm. I have seen people waste months trying to get soluble, active eukaryotic enzymes from E. coli when switching to a baculovirus or yeast expression system would have solved the problem in a few weeks.
Regulation and Nuance Beginners Miss
Translation is heavily regulated at every stage. In eukaryotes, the phosphorylation state of eIF2 controls global translation rates during stress responses. When eIF2 is phosphorylated, it binds eIF2B tightly and cannot be regenerated, effectively shutting down most protein synthesis. This is a key part of the integrated stress response. It is not a failure mode. It is a deliberate downregulation that conserves resources during adverse conditions. Internal ribosome entry sites, or IRES elements, allow certain mRNAs to initiate translation without a 5' cap. This is how some viral mRNAs and a subset of cellular mRNAs bypass the normal cap-dependent regulation. Under conditions where cap-dependent translation is suppressed, IRES-mediated translation can continue. This is clinically relevant because it means some stress-response genes keep getting translated even when most cellular protein synthesis is shut down. Another thing that is rarely emphasized is that translation and transcription are coupled in prokaryotes. The ribosome begins translating an mRNA while it is still being synthesized by RNA polymerase. This has consequences for gene regulation, mRNA stability, and even the timing of folding events. In eukaryotes, the nuclear envelope separates these processes, which adds a layer of regulation but also introduces transport bottlenecks.
Practical Considerations and Limitations
If you are working with this mechanistically, whether in a research or biotech context, there are a few practical realities worth noting. Codon optimization is useful but not a silver bullet. Over-optimizing can actually reduce expression by eliminating regulatory pauses that are needed for proper folding. I have seen codon-optimized constructs that expressed at half the yield of the original sequence simply because the ribosome was pushing through too fast and the protein aggregated. Leader sequences matter more than people tend to appreciate. The 5' untranslated region of an mRNA can contain structures and motifs that regulate translation efficiency. Adding a simple leader sequence derived from a highly expressed gene can improve translation rates substantially in both prokaryotic and eukaryotic systems. The exact effect depends on your system, but it is usually worth testing as a variable rather than assuming your construct will translate efficiently by default. The biggest limitation of standard translation machinery in recombinant systems is that it does not always produce homogeneous products. Alternative start sites, stop codon readthrough, frameshifting, and incomplete termination can all generate variant proteins from a single transcript. If you need a single defined product, you have to verify the N and C termini experimentally, usually through mass spectrometry or Edman degradation. Assuming the sequence implies the product is a common mistake.
In Vivo translation fidelity can also be affected by environmental factors. Temperature shifts, osmotic stress, and nutrient limitation all influence elongation rates and error rates. If you are doing structural biology and need homogeneous samples, keeping your expression conditions extremely stable matters more than the specific vector or strain you choose. Small fluctuations in growth temperature can shift the product distribution in ways that are hard to detect until you are trying to crystallize or analyze your protein.