The Basic Mechanics of Passive Molecular Movement
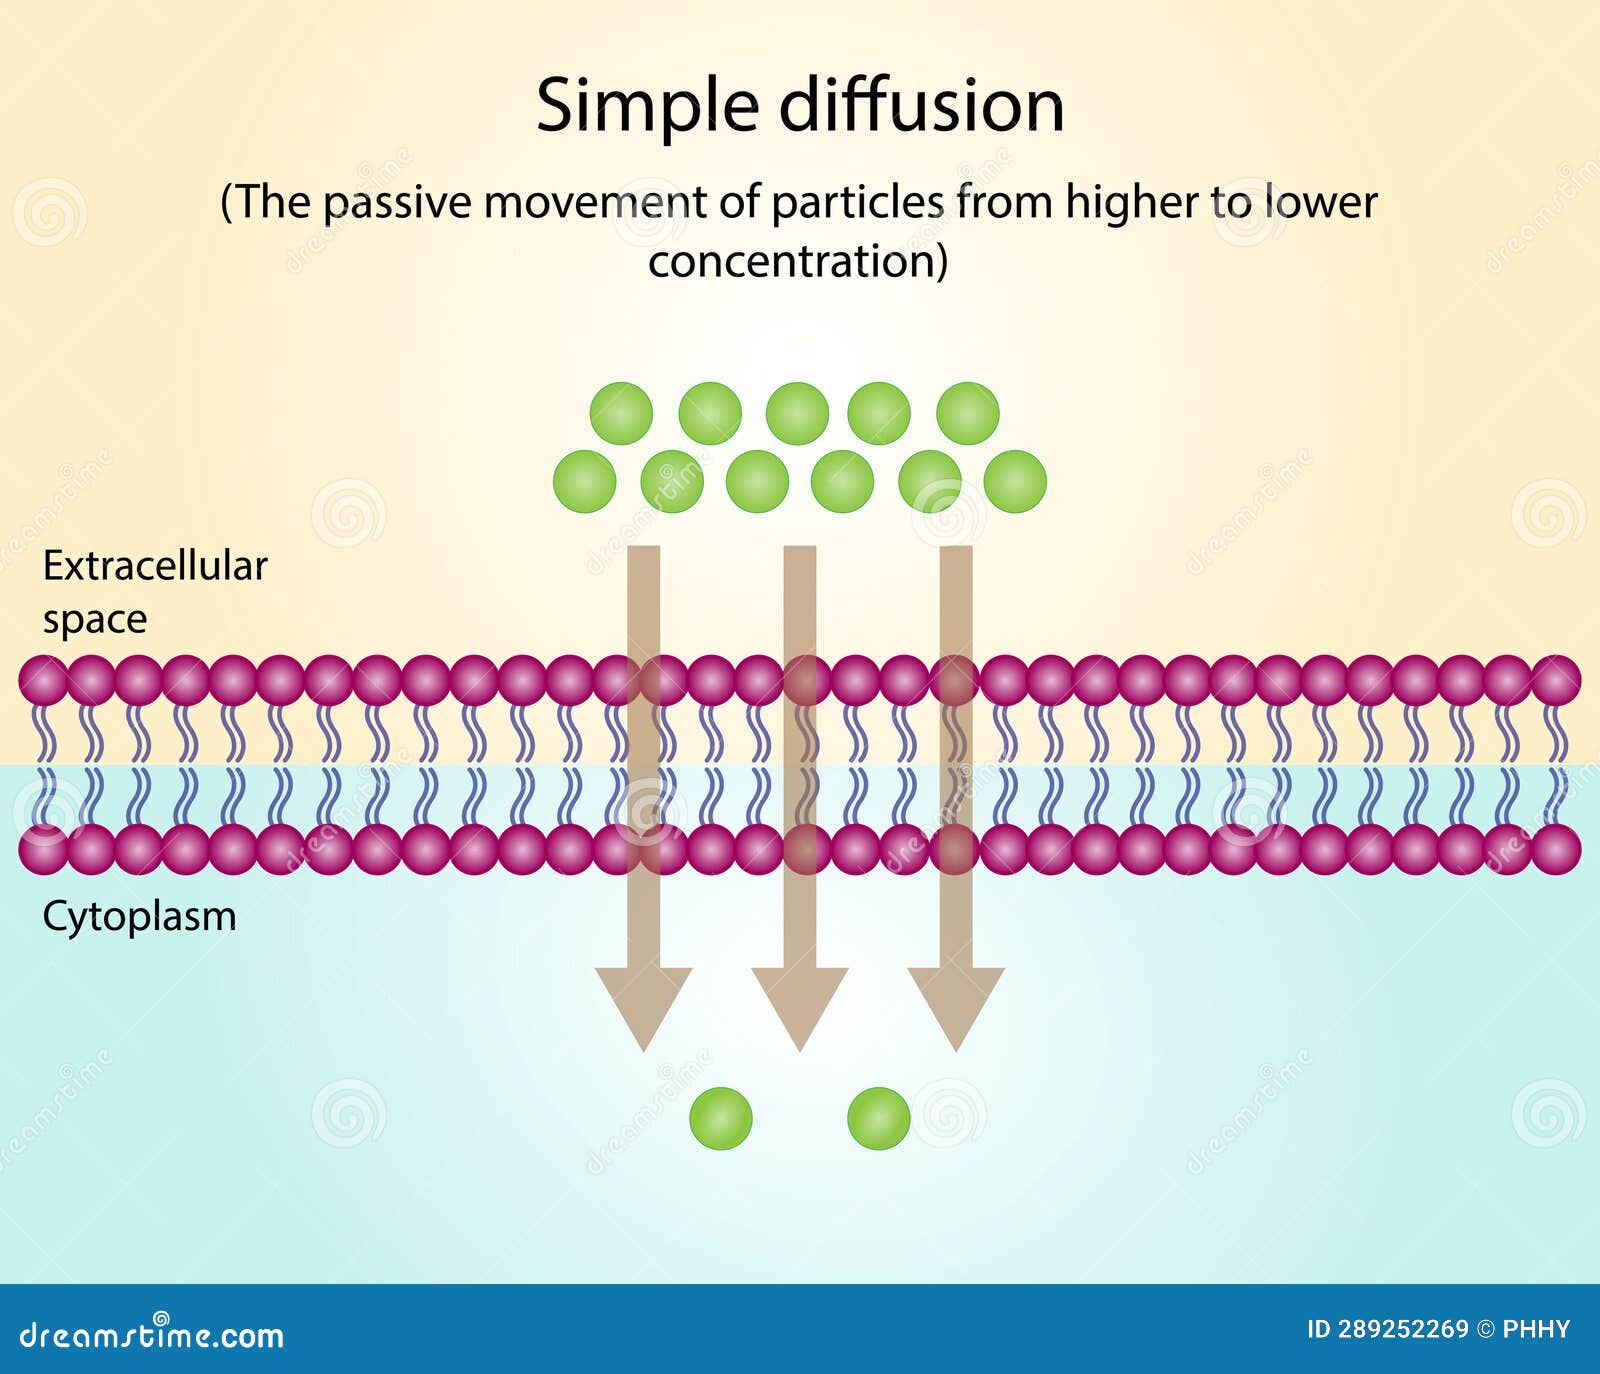
Simple diffusion is the process where small, nonpolar molecules move directly through a lipid bilayer without any protein assistance, following their concentration gradient until equilibrium is reached. It sounds straightforward because it is, but the details matter more than most introductory courses let on. I spent way too many hours troubleshooting why certain compounds wouldn't cross synthetic lipid membranes in our lab experiments, and the answer almost always came down to basic simple diffusion principles that most people gloss over. You have a concentration difference on either side of a membrane. Molecules move from high concentration to low concentration. That's the whole mechanism. No ATP. No channel proteins. Just thermal motion doing its thing. The rate at which this happens depends on several factors that compound together. Temperature increases kinetic energy and speeds things up. The surface area of the membrane matters—a larger area means more molecules can cross simultaneously. The concentration gradient itself drives the process, though the relationship isn't linear across all conditions. And the permeability of the membrane to a given molecule determines whether it can slip through the lipid bilayer at all.
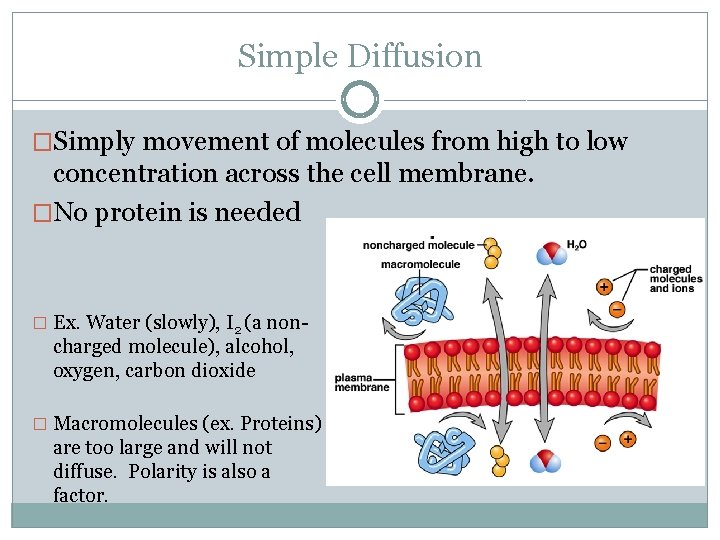
Small uncharged molecules like oxygen and carbon dioxide move through effortlessly. They're hydrophobic enough to dissolve into the lipid interior and diffuse across without any help. Lipid-soluble vitamins and steroid hormones work the same way. I once had a student who couldn't figure out why ethanol crossed cell membranes so much faster than glucose despite both being small molecules. The difference is polarity and size relative to the hydrophobic core. Ethanol is small and partially lipid-soluble. Glucose is hydrophilic and simply cannot penetrate the bilayer on its own.
What Beginners Get Wrong About This Process
Most people think concentration gradient is the only thing that matters. It isn't. Membrane composition plays a massive role that gets ignored constantly. A membrane rich in cholesterol is less permeable to small molecules than one without it. The cholesterol packs between phospholipid tails and reduces free volume within the bilayer. Saturated fatty acid chains also pack tighter than unsaturated ones, making the membrane more ordered and less permeable. Temperature shifts can flip this entirely—cool a membrane below its phase transition temperature and it becomes gel-like and nearly impermeable to diffusion. Another misconception is that diffusion stops at equilibrium. It doesn't stop. Molecules keep moving in both directions equally. That's dynamic equilibrium. The net flux is zero, but individual molecules are still crossing back and forth constantly. I've seen people misinterpret flat lines on a concentration-over-time graph as molecules coming to rest, which they never do. The math behind this is Fick's laws, but you probably don't need the full derivation. The practical takeaway is that flux is proportional to the concentration gradient and the permeability coefficient. Double the gradient and you double the flux, assuming everything else stays constant. That changes if the permeability coefficient itself shifts with temperature or membrane composition.
Get the Full Details
Where Simple Diffusion Breaks Down Completely
Here's the thing nobody tells you: simple diffusion is only useful for a very narrow range of molecules. If you're working with ions, polar molecules, or anything larger than about 100 daltons, simple diffusion through a lipid bilayer is essentially negligible. The rate becomes so slow it's biologically irrelevant. That's why cells evolved transport proteins. Not because simple diffusion is inadequate for every substance, but because it only works for a specific subset and living systems need to move plenty of things outside that subset. I remember running assays where we measured the permeability of various drugs across artificial membranes. Some compounds that looked promising in vitro fell apart completely because their simple diffusion rates were orders of magnitude too slow. A drug might bind its target with nanomolar affinity, but if it can't cross the membrane fast enough to reach intracellular concentrations, that affinity is useless. We found that adding a methyl group to certain polar compounds would dramatically increase their permeability. Even a small increase in lipophilicity can shift a molecule from nearly impermeable to reasonably permeable. It's a subtle effect that takes real experimental work to quantify properly. There's also the issue of membrane asymmetry. Real biological membranes aren't symmetric mixtures. The inner and outer leaflets have different lipid compositions, which affects local permeability in ways that symmetric model membranes can't capture. If you're doing research that requires accurate permeability measurements, standard liposomes made from a single lipid blend will give you data that looks clean but doesn't reflect what actually happens in a real cell.
Simple diffusion also can't explain directed transport. When a cell needs to accumulate a substance against its gradient, simple diffusion does exactly the opposite—it equalizes concentrations. Active transport mechanisms exist precisely because the passive process alone can't handle those situations. Don't try to fit every membrane transport problem into a diffusion framework. It won't work. The practical applications span from drug design to understanding gas exchange in lungs and gills. In the alveoli, oxygen diffuses across a membrane that's approximately 0.5 micrometers thick. Carbon dioxide moves about 20 times faster than oxygen across the same barrier because it's more soluble in lipids despite being a larger molecule. Solubility often matters more than molecular weight when we're talking about simple diffusion through a lipid phase.


