The Role of Consumers in Ecosystems
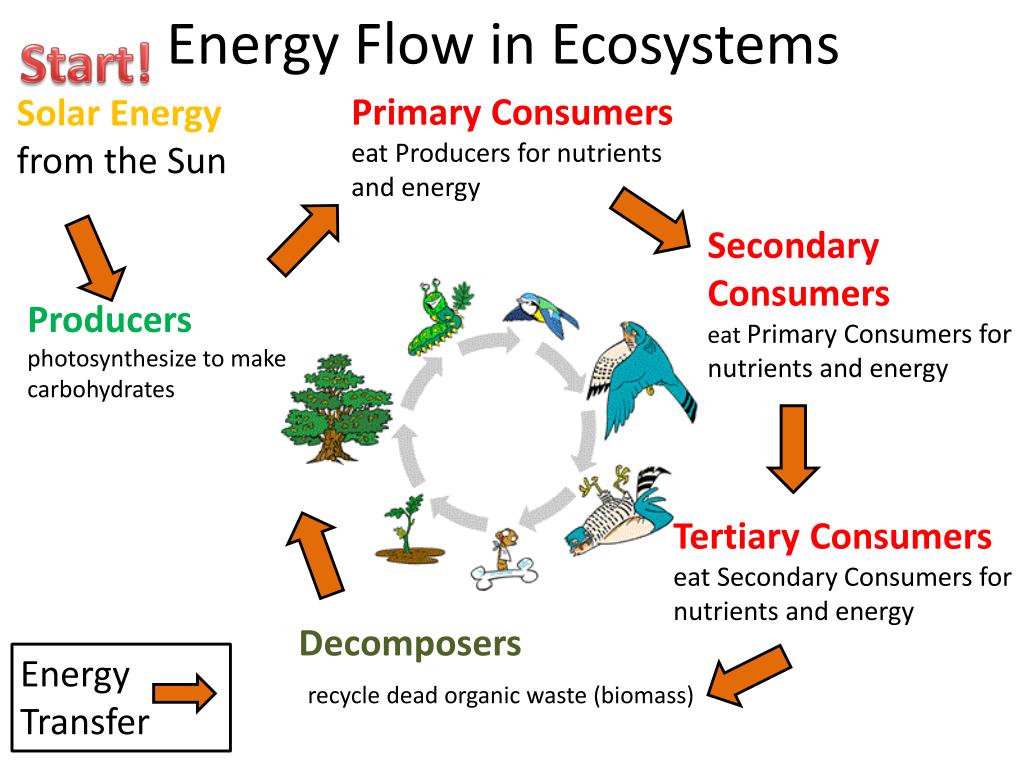
A consumer in ecology is any organism that obtains energy by eating other organisms or organic matter, rather than producing its own food through photosynthesis or chemosynthesis. That basic definition covers everything from the rabbit grazing on grass to the fungus decomposing a fallen log. Consumers drive energy flow through ecosystems, moving sunlight-derived energy from producers up through increasingly specialized feeders until it eventually dissipates as heat. I have worked on grassland and forest edge sites for over a decade, and one thing becomes clear fast: consumers are not just passive energy transfers. They are the engineers of population dynamics, nutrient cycling, and physical habitat structure. A single overabundant herbivore can strip vegetation, change soil chemistry, and trigger cascading effects that reach microbial communities and bird nesting success. The energy that flows through a consumer network determines how much biomass the system can support at every level. Understanding this concept correctly matters because many people confuse consumers with predators alone. Predation is only one consumer strategy. Grazing, browsing, detritivory, parasitism, and decomposition are all consumer pathways, and each has different consequences for energy distribution.
What Is A Consumer In Ecology The Vital Players In Energy Flow Across Ecosystems
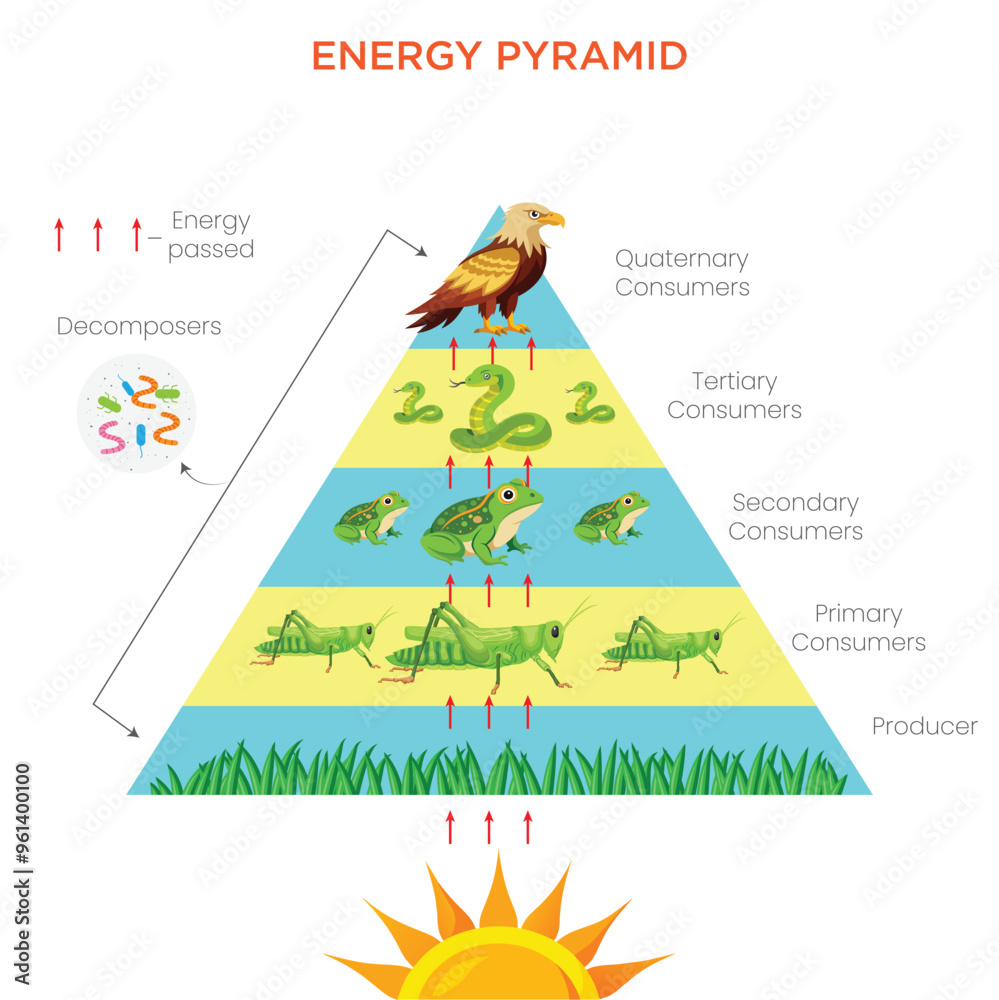
The title phrase captures the core idea: consumers are the vital players that move energy through ecosystems. Without them, primary production would accumulate as standing biomass and rarely reach higher trophic levels. Nutrients would remain locked in dead tissue longer, decomposition rates would drop, and system productivity would collapse over time. Consumers create the throughput that keeps ecosystems functioning dynamically. Here is how consumer classification actually works in practice. Ecologists divide consumers mainly by diet and trophic position. Primary consumers eat producers, which means herbivores in most terrestrial systems. Secondary consumers eat primary consumers, which makes them carnivores or omnivores that prey on herbivores. Tertiary and quaternary consumers occupy the top of food chains, feeding on other carnivores. Detritivores consume dead organic material, while decomposers break down that material chemically and biologically. Parasites and parasitoids are consumers too, drawing energy from living hosts without immediately killing them. When I teach field methods, I always start with trophic level mapping because it forces students to see the links instead of memorizing categories. You identify the producers in a plot, then list the primary consumers using plant tissue or excrement evidence, then track secondary consumers through direct observation, scat, or prey remains. That process reveals gaps and unexpected links. In one study site, we assumed insectivorous birds were secondary consumers, but stable isotope work showed they were pulling significant energy from tertiary sources by eating parasitoid wasps that attacked herbivorous caterpillars. That shifted our entire energy budget model.
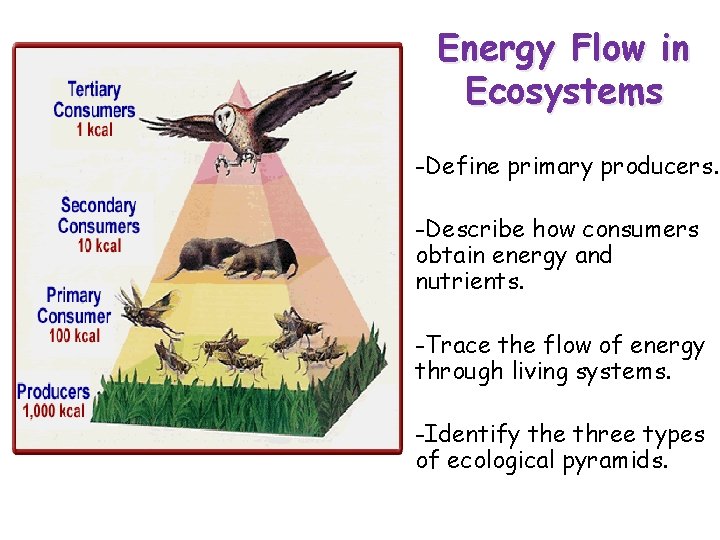
Energy transfer efficiency is a central practical issue. The textbook ten percent rule is a rough average, not a hard law. Real transfers range from about five to twenty percent depending on organism type, temperature, and trophic step. In cold aquatic systems, energy transfer can be slightly more efficient because metabolic costs drop. In hot terrestrial systems, respiration losses are higher, so less energy moves to the next level. That variation explains why food chains rarely exceed four or five steps. By the time you reach a top predator, most of the original solar energy captured by producers is gone, lost as heat through metabolism and incomplete digestion. I ran into a specific problem once while modeling a temperate stream food web. We measured algal biomass, grazers, and fish, but our energy flow estimates were off by nearly forty percent. The issue turned out to be microinvertebrate detritivores that we had not sampled adequately. They were processing leaf litter and fine particulate organic matter at rates that fed the benthic community and subsidized the fish population. Adding a detrital pathway corrected the model and doubled the estimated energy available to secondary consumers. If you skip detritivores and decomposers, you will consistently underestimate consumer-driven energy flow. Consumer functional groups also matter beyond trophic position. Keystone consumers exert disproportionate influence relative to their biomass. Sea otters are the classic example, controlling sea urchin populations and thereby protecting kelp forests. Without otters, urchins graze kelp to the holdfasts, converting productive habitat into barren zones. That shift reduces energy available to dozens of associated species. In freshwater systems, large piscivorous fish can regulate midlevel predators, which then changes zooplankton grazing pressure and algal biomass. These cascades are consumer effects, not just population effects.
Get the Full Details
Another practical point is that consumers respond to environmental variation, and that response shapes energy flow. Temperature, moisture, and nutrient availability alter consumer metabolism and feeding rates. In warming climates, many consumer populations increase their respiration demand before they increase intake, which can reduce growth efficiency. That means less energy is converted into biomass at each trophic level, and more is lost as heat. For ecosystem modelers, that is a critical detail. Assuming constant conversion efficiency across warming scenarios will overestimate higher trophic biomass. Decomposers and detritivores deserve separate emphasis even though they are consumers. Fungi, bacteria, earthworms, millipedes, and many insect larvae process dead material and release nutrients for producers. They close the loop. Without them, energy captured by photosynthesis would remain trapped in dead tissue, and nutrient recycling would slow dramatically. In boreal forests, slow decomposition under cold, acidic conditions means organic matter accumulates for decades. In tropical rainforests, rapid decomposition returns nutrients quickly, and most biomass is held in living plants rather than soil. Consumer-driven decomposition rates are therefore a major determinant of ecosystem carbon storage. Parasites are consumers too, and they are often ignored in introductory treatments. Parasites can regulate host populations, alter host behavior, and create energy sinks that redirect flow away from higher predators. A common parasitic trematode in snails castrates the host and redirects energy from reproduction to parasite growth. That change affects how much energy the snail community contributes to fish predators. Ignoring parasites in food web models can produce misleading energy flow predictions, especially in aquatic systems where parasitic diversity is high.
If you want to study consumers in a hands-on way, start small and be systematic. Pick a defined patch of habitat, map the plant species, and then record the herbivores feeding on them over multiple seasons. Note time of day, temperature, and plant part consumed. Then look for predators of those herbivores. Scat analysis, prey remains, and direct observation all work, but each has limits. Scat tells you what was eaten recently, not long-term diet. Prey remains indicate predation events but not consumption rates. Direct observation is accurate but time-intensive and weather-limited. Stable isotope analysis is a powerful tool for consumer ecology, though it requires laboratory access. Carbon and nitrogen isotope ratios reveal trophic position and carbon sources over weeks to months, depending on tissue turnover. I have used this method to show that seemingly terrestrial birds in riparian zones were feeding primarily on aquatic insects, which shifted our understanding of energy flow between ecosystems. That cross-habitat subsidy effect is common but easily missed without isotopic data. One limitation to acknowledge is that consumer definitions and classifications can blur in complex systems. Omnivory is widespread, and many species occupy multiple trophic positions simultaneously. That makes simple linear food chains inadequate for describing real energy flow. Food webs capture that complexity better, but they also become harder to parameterize with empirical data. If you are building a model, consider using a range of trophic positions rather than fixed levels, and test how sensitive your energy flow estimates are to those assumptions.
Another pitfall is assuming consumer biomass always tracks resource availability closely. There are often time lags, numerical responses, and density-dependent effects that decouple consumer and resource dynamics. In predator-prey cycles, consumer peaks follow resource peaks by months or years. Misinterpreting that lag as a lack of connection leads to wrong conclusions about energy flow. Long-term data sets are essential for separating correlation from causation in consumer-resource relationships. From a management perspective, consumer conservation is often the most effective lever for ecosystem restoration. Reintroducing wolves to Yellowstone is a famous example, but smaller-scale consumer interventions also work. Restoring native pollinators increases plant reproductive success and alters energy flow toward seed production. Protecting detritivore communities accelerates nutrient cycling in degraded soils. Removing invasive consumers that lack natural predators can prevent trophic cascades that degrade habitat quality. Each intervention changes energy pathways, sometimes in ways that are hard to predict fully. The takeaway is straightforward but important. Consumers are not optional add-ons to ecosystems. They are the mechanisms that distribute energy, regulate populations, and cycle nutrients. Their diversity and abundance determine how resilient a system is to disturbance and how efficiently it converts primary production into higher trophic biomass. Studying them requires attention to trophic links, detrital pathways, and environmental context. Ignoring any of those elements produces an incomplete picture of energy flow.

What Is A Consumer In Ecology The Vital Players In Energy Flow Across Ecosystems is ultimately a question about connectivity. Consumers connect producers to decomposers, link habitats through mobility, and translate solar energy into biological form that supports complex communities. That role is fundamental, measurable, and increasingly important as human activities alter consumer populations worldwide. The mechanisms are well understood, but applying that understanding consistently across diverse ecosystems remains the ongoing challenge.

.png/1766065745.png "Energy Flow In Ecosystem, Food Web, Ecological Pyramids, More, UPSC Notes")