Understanding Genetic Shuffling in Meiosis
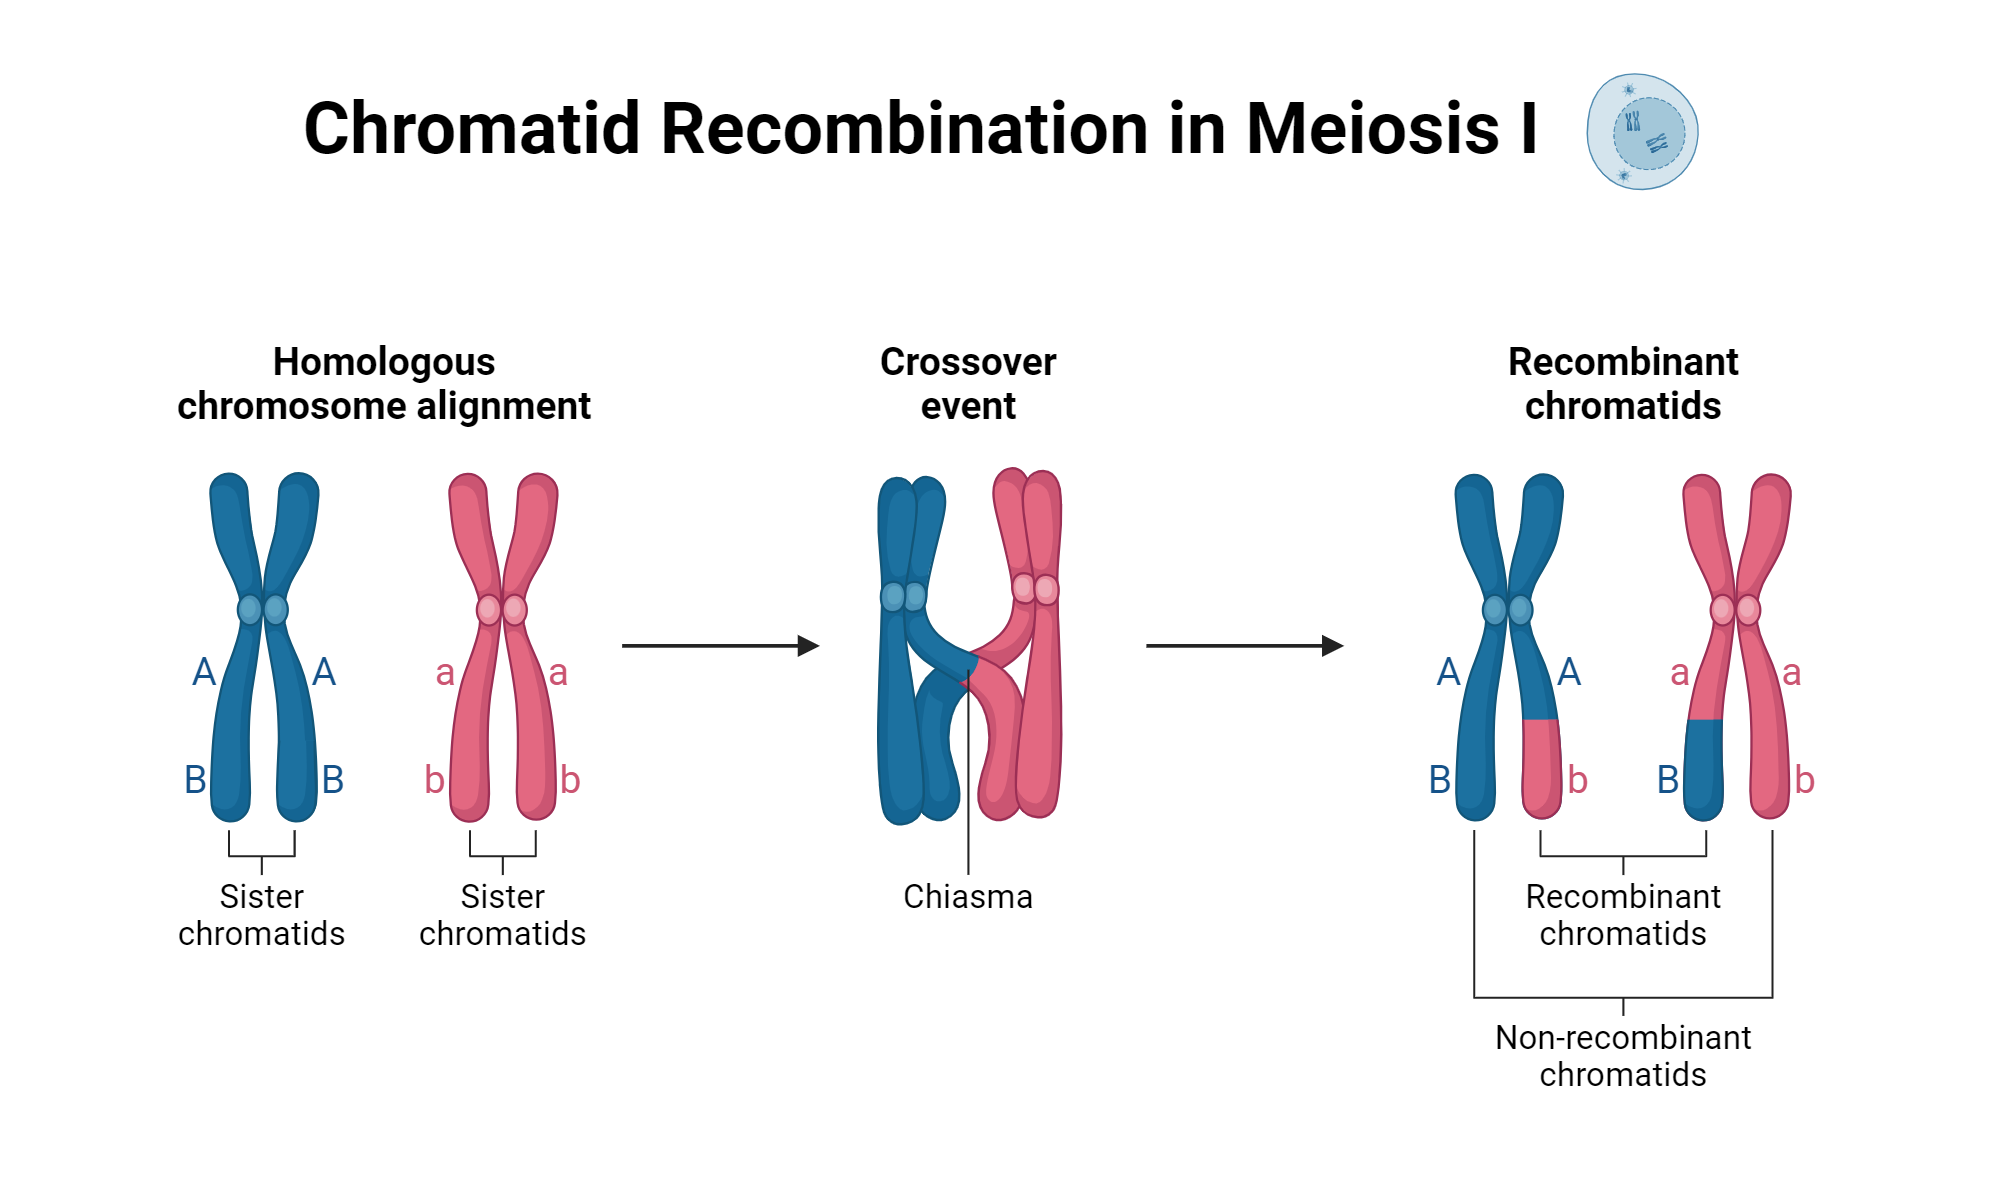
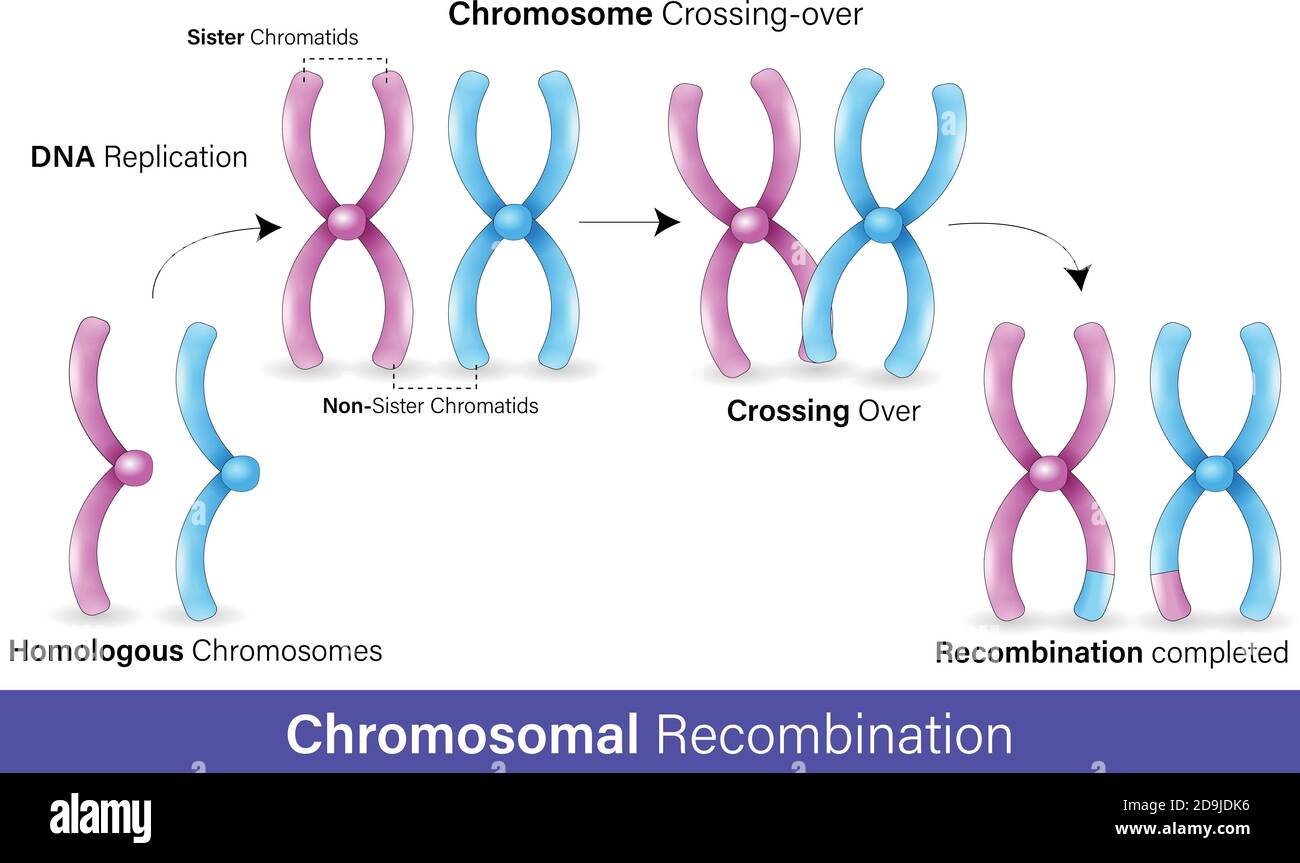
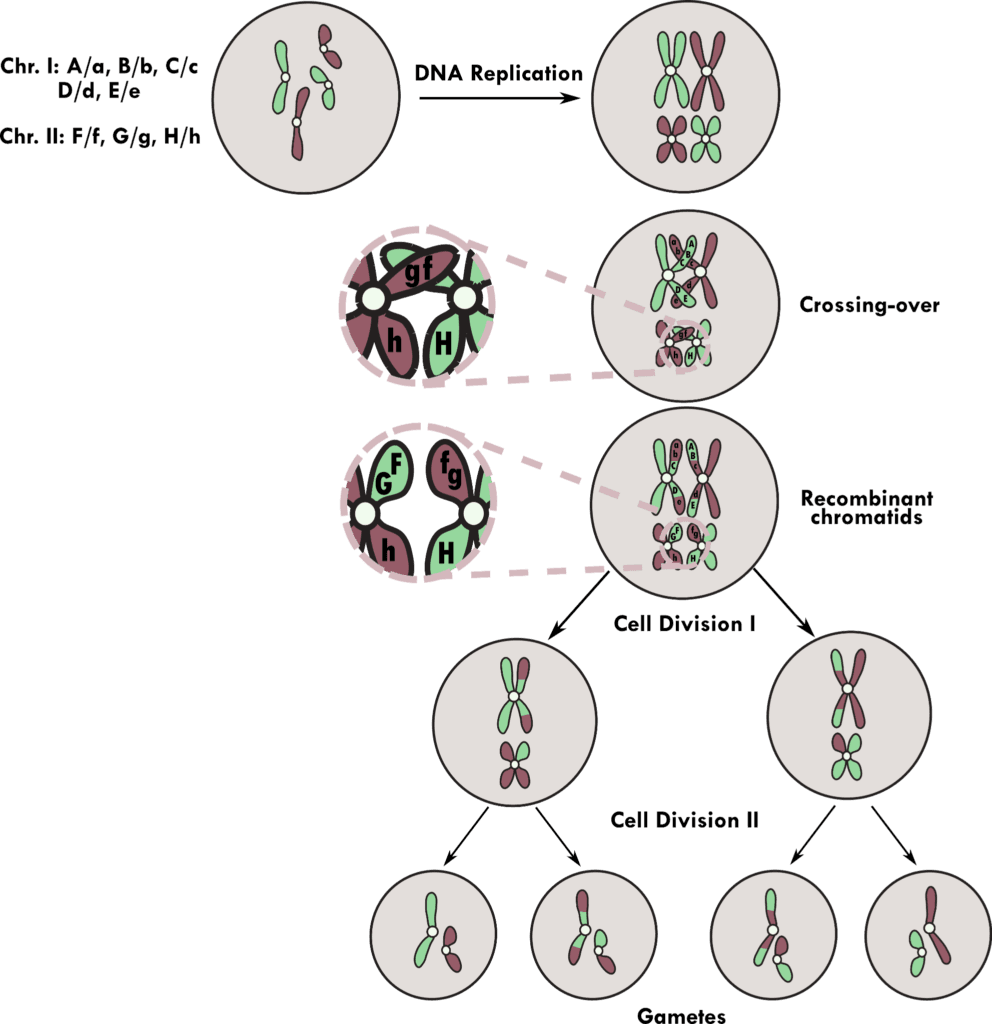
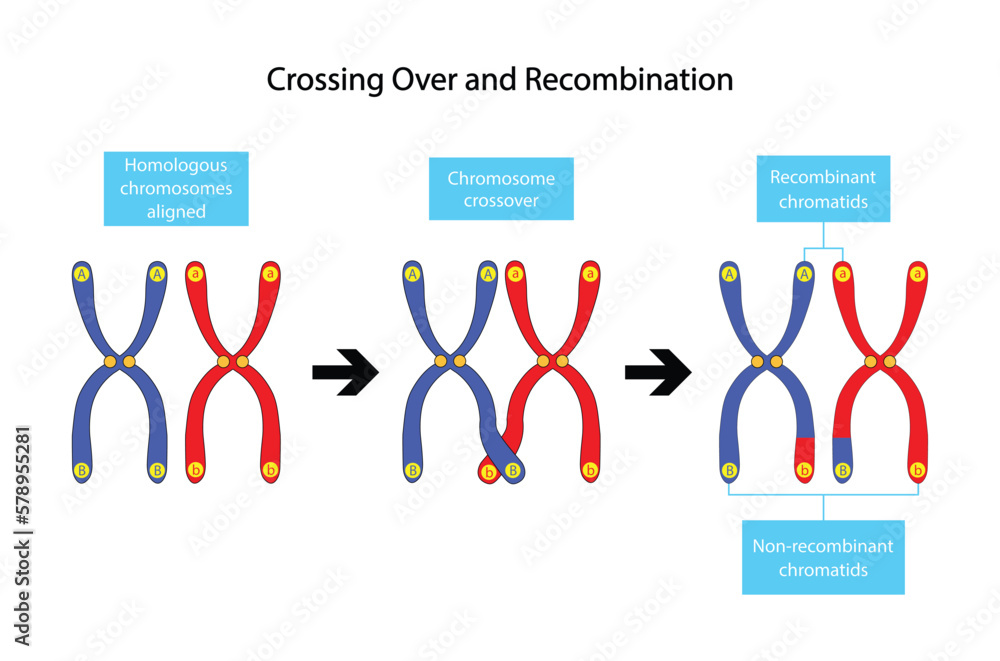
Meiosis is the process where diploid cells divide to create gametes, and recombination is the mechanical act of swapping DNA between homologous chromosomes. This happens during prophase I when chromosome pairs line up and physically exchange segments. The result is that every sperm and egg carries a unique combination of genetic material from both parents, not just intact copies of the original chromosomes. The advantages are largely about variation. When genes get shuffled, offspring end up with novel allele combinations that neither parent had as a complete package. This matters for evolution because it gives natural selection more raw material to work with. Populations with higher recombination rates adapt faster to changing environments since beneficial mutations can be brought together without waiting for separate mutation events to occur in the same lineage.
What Are The Advantages Of Recombination During Meiosis How Shuffling Genes Fuels Evolution And Health
From a health perspective, recombination helps purge deleterious mutations. In asexual organisms, harmful mutations accumulate irreversibly over generations—a problem known as Muller's ratchet. Recombination allows chromosomes carrying fewer mutations to be selected against chromosomes carrying more, effectively giving populations a way to shed genetic load. For vertebrate immune systems specifically, the shuffling of MHC region alleles through recombination produces individuals capable of recognizing a broader range of pathogens, which directly correlates with disease resistance at the population level. The molecular mechanics involve programmed double-strand breaks catalyzed by the SPO11 enzyme. These breaks are repaired using the homologous chromosome as a template, and depending on how the repair resolves, you get either a crossover event where flanking markers are exchanged or a non-crossover gene conversion event where only a small patch of sequence is copied over. Crossovers are also mechanically necessary—they create chiasmata, the physical connections that hold homologous chromosomes together so they orient correctly on the metaphase plate. Without crossovers, chromosomes segregate randomly and aneuploidy rates spike dramatically. That is why organisms with severely reduced recombination, like male Drosophila, still manage viable gametogenesis through alternative stabilization mechanisms. I ran into a practical problem a few years ago mapping a trait in a model organism and finding recombination frequencies that made no sense by standard genetic map expectations. The locus I was tracking sat near a known recombination hotspot, but the hotspot activity was highly variable between individuals due to a polymorphism in the PRDM9 binding motif. This meant that two crosses that should have produced identical mapping resolution were producing wildly different confidence intervals on the positional clone. The workaround was straightforward once I identified the issue: I genotyped the parents for the PRDM9 allele, selected heterozygous crosses where the hotspot was active in the recombinant background, and used those progeny exclusively for fine mapping. It cut the mapping window from roughly 2 megabases down to about 80 kilobases in a single experiment, whereas standard approaches would have required dozens of additional backcrosses to achieve the same resolution.
There are real costs to recombination that get glossed over in introductory biology courses. Crossovers are not uniformly distributed across the genome. In humans, about 60 percent of crossovers fall within the top 10 percent of recombination hotspots, leaving vast genomic regions with very low exchange rates. This means linkage disequilibrium persists over long distances in cold regions, making it harder to separate linked causal variants from nearby markers. It also means certain combinations of alleles never get broken apart, which can trap deleterious mutations alongside beneficial ones—a phenomenon called background selection. Recombination can also go wrong. Ectopic recombination between repetitive sequences on non-allelic positions causes deletions, duplications, and inversions. Most of these structural variants are either neutral or slightly deleterious, but a significant fraction causes disease. Recurrent deletions at loci like 17p12 cause Charcot-Marie-Tooth disease type 1A through exactly this mechanism, and the breakpoints trace back to low-copy repeats that facilitate misalignment during meiosis. The recurrence rate for these disorders is surprisingly high precisely because the underlying sequence architecture makes recombination errors somewhat predictable rather than purely random. Another thing beginners miss is the assumption that more recombination is always better. There is a well-documented tradeoff. While recombination generates beneficial diversity, each crossover event carries a risk of mis-segregation if the chiasmata do not resolve properly. Organisms in stable environments often show reduced recombination rates, and stress can actually suppress recombination in some species rather than increase it. The relationship between recombination rate and fitness is not linear—it follows a curve where moderate rates optimize the balance between adaptive potential and segregation fidelity.
Get the Full Details

The energy cost is another constraint. Meiotic recombination requires extensive protein machinery including the cohesin complex, the synaptonemal complex, and multiple recombinase enzymes. Errors in this machinery are a leading cause of infertility and miscarriage in humans. Aneuploid pregnancies, particularly trisomy 21, are strongly correlated with advanced maternal age and correlate with altered recombination patterns in oocytes—not simply fewer crossovers but crossovers placed in suboptimal positions on the chromosome arm. This is why prenatally detected aneuploidy patterns follow such consistent chromosomal signatures across populations. Population-level data from the 1000 Genomes Project and more recent pangenome studies show that recombination rate variation itself is heritable and under selection. Regions of the genome with consistently high recombination tend to have lower nucleotide diversity because selective sweeps are more efficient at removing linked neutral variation. Conversely, low-recombination regions like centromeres and telomeres accumulate more repetitive DNA and transposable elements because selection is less effective at purging them. These patterns are visible in every sequenced vertebrate genome and represent a nearly universal signature of recombination's influence on genome architecture. Practical applications of understanding these mechanisms span medical genetics, conservation biology, and agricultural breeding. In conservation, populations with historically low recombination rates due to bottlenecks show elevated runs of homozygosity and reduced ability to respond to novel pathogens. In breeding programs, manipulating recombination rates through targeted hotspot activation or suppression has been used to accelerate the pyramiding of resistance genes in crops, though this remains an active area of research rather than routine practice. The key takeaway is that recombination is not just a source of randomness—it is a regulated, sequence-influenced process with predictable biases that can be leveraged when you understand the underlying constraints.