The Real Mechanics Behind How Single-Celled Organisms Split
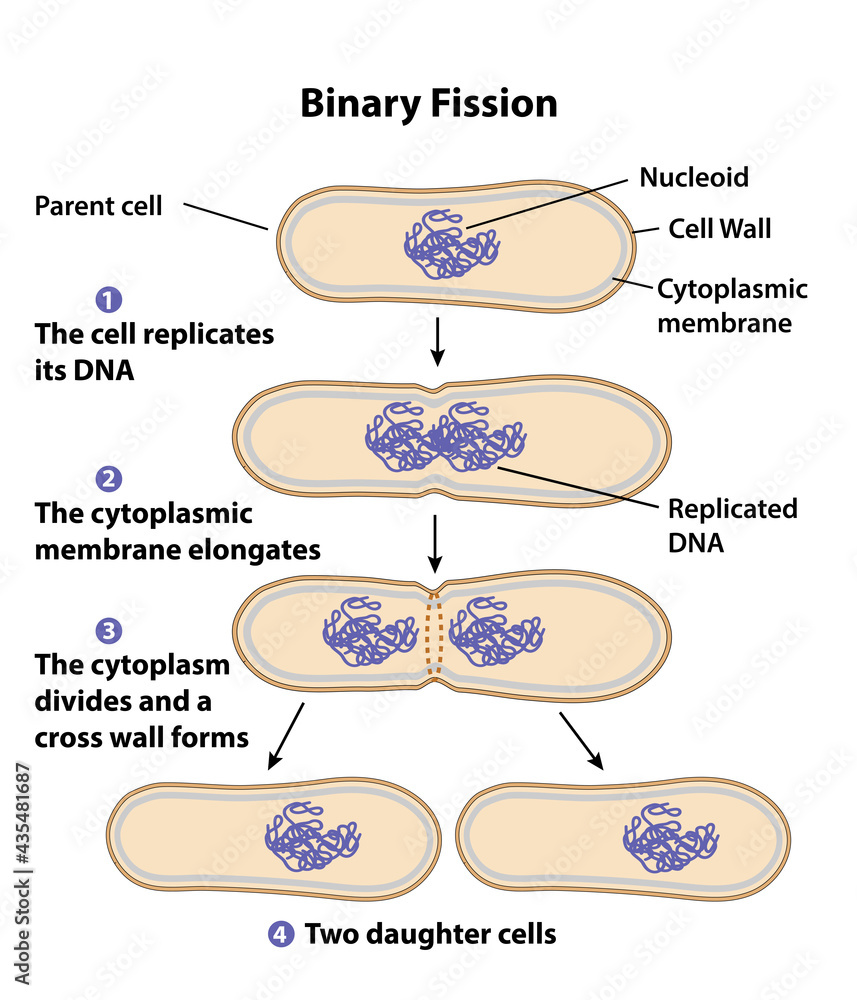
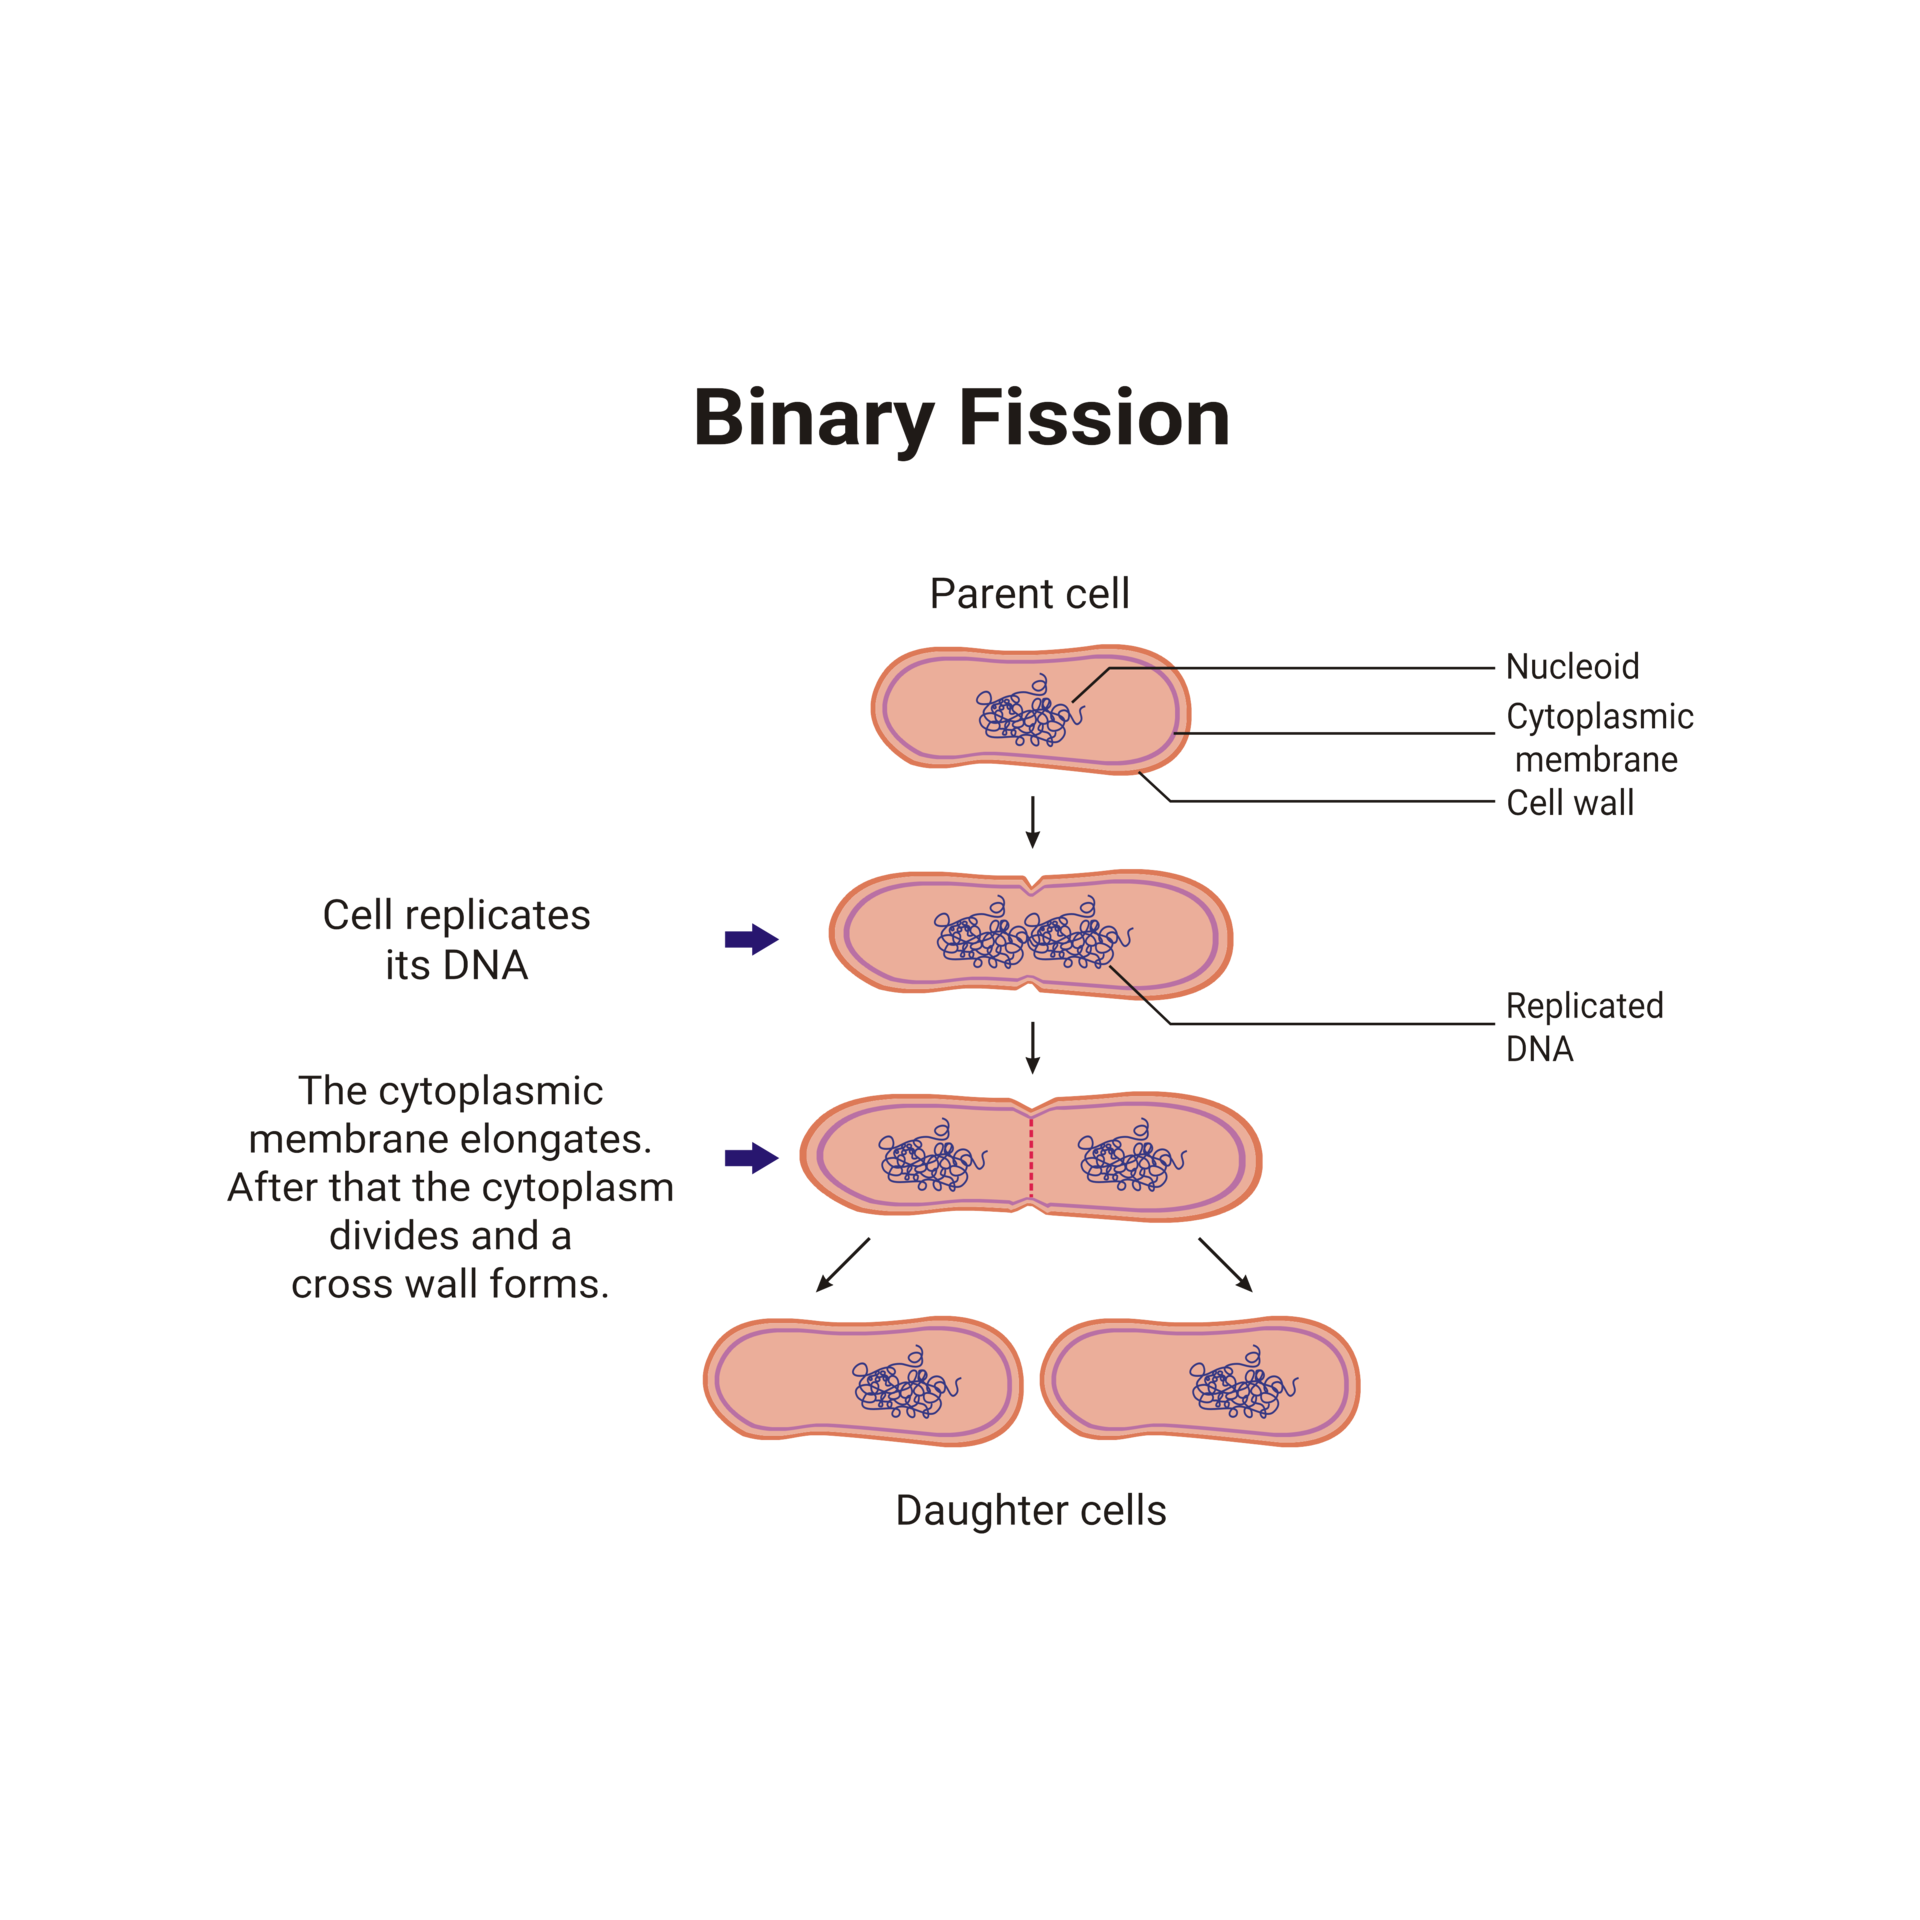
Binary fission is the method most prokaryotes use to reproduce, and honestly, it's far less elegant than textbooks make it sound. You've probably seen the diagram: one circle becomes two identical circles. That's the simplified version. The actual process involves coordinating DNA replication, membrane synthesis, and cell wall construction in a sequence that frequently goes wrong under suboptimal conditions. I've spent years working with bacterial cultures in teaching labs, and the difference between a clean fission event and a botched one usually comes down to growth medium quality and temperature stability. Before you get into the steps, you need to understand what makes this different from eukaryotic mitosis. Prokaryotes don't have a nucleus. Their single circular chromosome floats in the cytoplasm. There are no spindle fibers pulling chromosomes apart. The whole apparatus is simpler, but simpler doesn't mean more reliable. When I first started running E. coli cultures, I assumed binary fission would give me consistent doubling every 20 minutes under ideal conditions. My colony counts didn't match the math for three weeks straight. Turns out my incubator had a 2-degree temperature fluctuation that I couldn't see on the digital readout. That fluctuation was enough to slow replication and create elongated cells that hadn't completed septation. I ended up using a water bath instead, and the numbers aligned immediately. The sequence starts with DNA replication at the origin of replication, called oriC in E. coli. The DnaA protein binds to the origin, unwinds the helix, and recruits the replisome. This happens before the cell even reaches a critical size. By the time the cell doubles its mass, you typically have two fully replicated chromosomes. The nucleoid doesn't just split randomly. Active partitioning systems, particularly the ParABS system in many species, ensure each daughter cell receives at least one copy of the chromosome. Without ParABS, you get anucleate cells at disturbingly high rates.
After the chromosomes are positioned, the FtsZ protein ring assembles at the future division site. FtsZ is a tubulin homolog, which is why antibiotics targeting eukaryotic microtubules sometimes show cross-reactivity with bacterial division. The Z-ring contracts, recruiting over a dozen other proteins that build the septum. Peptidoglycan synthases insert new cell wall material while hydrolases cleave the existing wall. This coordinated insertion-and-cleavage mechanism is where most bottlenecks occur. If the synthases outpace the hydrolases, the septum becomes thick and stubborn, producing filamentous cells. If the hydrolases run ahead, you get weak spots and cell lysis. The final step is cytokinesis. The septum closes, the two daughter cells separate, and each inherits a complete copy of the genome along with roughly half the cytoplasmic contents. In practice, cytoplasmic distribution is never perfectly equal. One daughter often gets slightly more ribosomes or protein aggregates. This asymmetry matters more than you'd think for stress resistance and persistence phenotypes.
Common Pitfalls And Where People Get It Wrong
Beginners usually treat binary fission as a purely mechanical process. It isn't. Environmental factors dominate the timing and fidelity. Nutrient availability controls the C-period, the time required for chromosomal replication. In rich media like LB broth, C is about 40 minutes regardless of how fast the cell divides. But in minimal media, C stretches to 80 minutes or more, and the cell can't complete a division cycle fast enough to keep up with nutrient accumulation. You'll see cells pile up without dividing, forming long filaments that confuse anyone doing quick microscopic counts. The fix is straightforward: match your medium to your expected growth rate and let the culture reach log phase before expecting clean fission. Another mistake is assuming all bacteria divide the same way. Some use asymmetric division. Caulobacter crescentus produces a motile swarmer cell and a sessile stalked cell in every cycle. Mycoplasma species lack a cell wall entirely, so they divide by budding rather than the classic septation model. Streptomyces grow as branching filaments and fragment into spores. If you're studying binary fission in a lab setting, know what organism you're working with before applying general principles.
Get the Full Details
Watching It Happen In Real Time
If you want to observe binary fission directly, phase-contrast microscopy works better than brightfield. The contrast between the dividing septum and the rest of the cell is significantly higher. Staining with DAPI or SYTO 9 for nucleic acids helps you confirm chromosome segregation. I recommend capturing time-lapse sequences at 30-second intervals for E. coli at 37 degrees Celsius. At that growth rate, visible septation takes about 20 to 30 seconds, so faster frame rates won't add much value and will just bloat your file sizes. Quantitative work requires counting viable cells over time. Plate counts remain the gold standard despite being slow. Flow cytometry gives you speed but can't distinguish live from dead cells without a viability dye. I've used both propidium iodide and SYTO 9 in combination with flow, and the correlation with plate counts was within 5 percent for healthy log-phase cultures. Once cultures enter stationary phase, the dye exclusion method breaks down because membrane potential drops, and you start counting stressed-but-viable cells as dead. That's a known limitation worth noting if you're doing any kind of growth curve analysis.
When Binary Fission Fails Completely
Antibiotics that target cell wall synthesis, like penicillin and other beta-lactams, essentially weaponize the septation process. They inhibit penicillin-binding proteins, which are the transpeptidases responsible for cross-linking peptidoglycan strands. Without functional PBPs, the septum can't form properly. The cells continue to grow and replicate DNA but can't divide. They become osmotically unstable and lyse. This is why beta-lactams are bactericidal rather than bacteriostatic. They don't just stop division; they cause the cell to burst. Conversely, antibiotics like quinolones target DNA gyrase and topoisomerase IV, which are essential for resolving the supercoiled DNA during replication. Blocked replication means no chromosome segregation, which means no fission. These drugs are effective but select for resistance mutations very quickly in monotherapy. Combination therapy reduces that risk significantly. There are also natural inhibitors. Some soil bacteria produce macrolides and other secondary metabolites that interfere with FtsZ polymerization. Zeocin and related compounds have been used in research specifically because they disrupt the Z-ring. Understanding these mechanisms is useful if you're designing experiments that require controlled inhibition of cell division.
What This Means For Practical Work
If you're maintaining a bacterial strain, the simplest rule is to keep cultures in mid-log phase for consistent division rates. Harvesting too late means stationary-phase cells that may not divide upon rep inoculation. Over-inoculating fresh medium causes the same problem because the carrying capacity is reached before true exponential growth begins. Seed at no more than 1 percent of the overnight culture into fresh medium and incubate with shaking at the optimal temperature for your organism. For anyone doing molecular cloning or protein expression, asynchronous division is actually an advantage. You want a mixed population so that when you induce expression, not every cell is in the same metabolic state. Inducing a perfectly synchronized culture often leads to uneven expression patterns because the entire population hits the stress response at the same time. A log-phase culture with natural division variability handles induction much better. The take-away isn't that binary fission is complicated. It's that the simplicity of the model obscures the regulatory complexity underneath. The core mechanism is conserved across most bacteria, but the timing, fidelity, and outcomes depend heavily on conditions that are easy to overlook in a standard lab protocol. Pay attention to those details and the process behaves predictably. Ignore them and you'll spend weeks chasing inconsistencies that have nothing to do with your experimental design and everything to do with a slightly off incubator temperature or a batch of medium that's been sitting too long.


