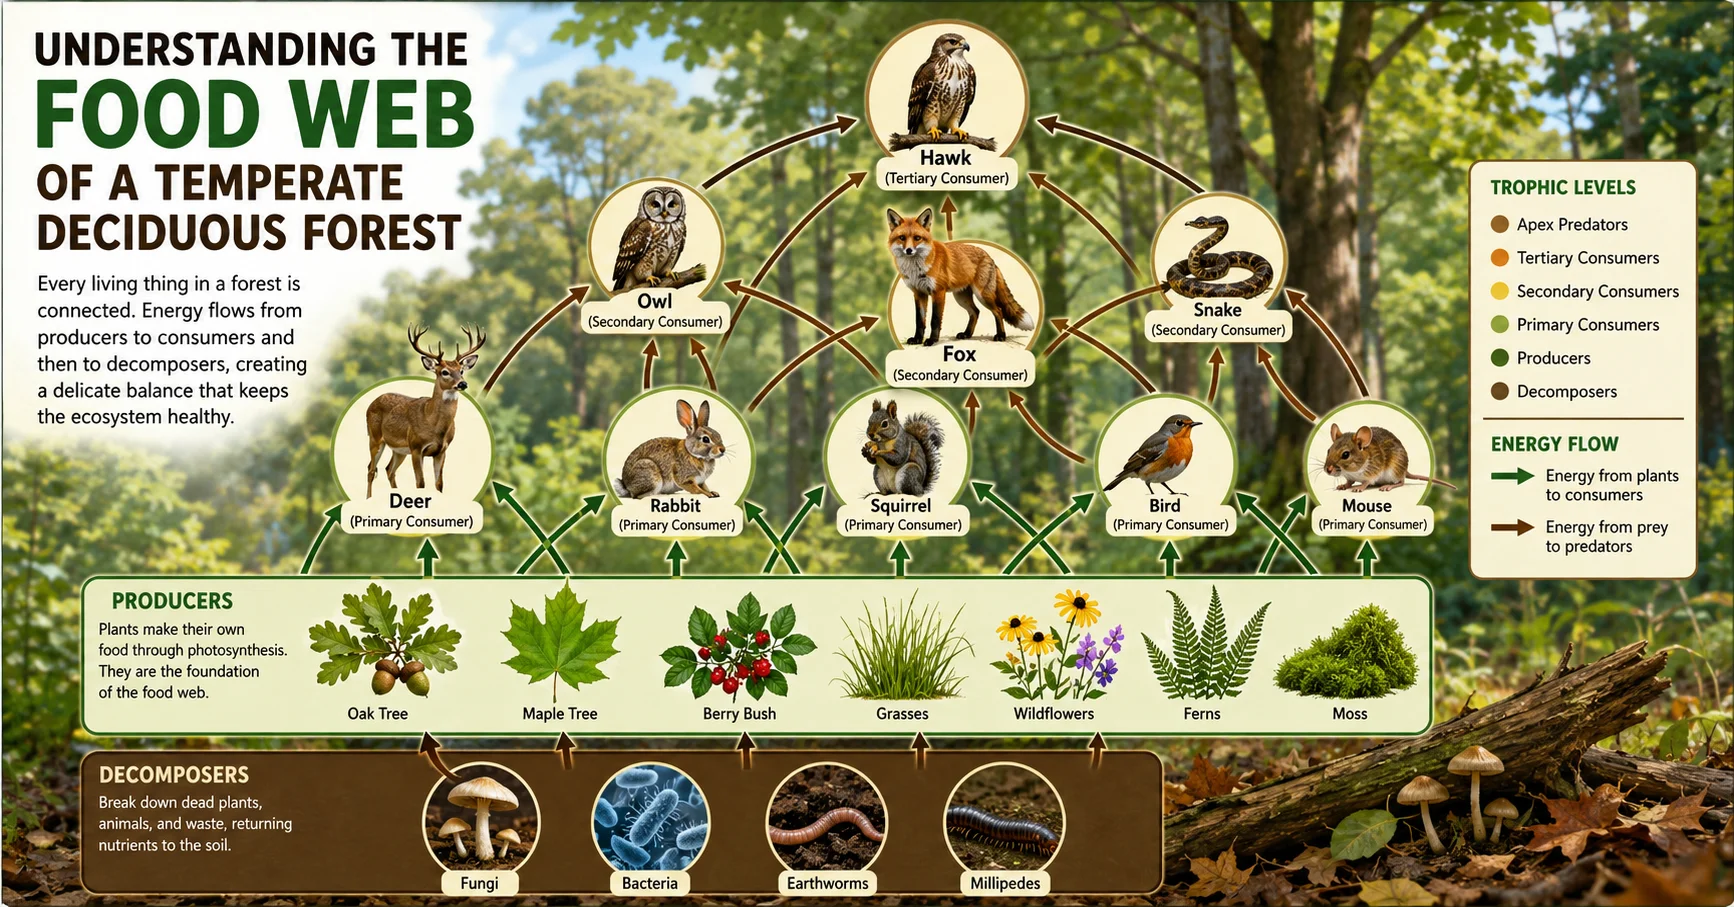
Mapping the Real Energy Flow in a Deciduous Forest
Most textbooks present the temperate deciduous forest as a simple chain: oak tree, caterpillar, chickadee, hawk. That's not wrong, but it's incomplete and it can mislead you when you're actually trying to understand how this ecosystem operates. The grazing food web — the one starting with photosynthesis in live leaves — matters. It's just not the main character in this story. The real powerhouse of a temperate deciduous forest is the detrital pathway, and it runs on leaves that have already fallen and died.I spent a stretch of fieldwork in a mixed oak-hickory forest in southern Indiana trying to map energy flow through that system. What I found was that approximately 90 to 95 percent of the energy consumed by organisms at the forest floor level came from dead leaf material, not from living plant tissue. The few herbivores that do eat live leaves — spring ephemeral specialists, certain beetle larvae — are a small side channel. The bulk of the biomass processing happens below ground and among the leaf litter. To actually understand this system, you need to track three distinct phases across the year. Phase one is autumn leaf fall and the early breakdown stage. Leaves drop between late September and early November depending on your latitude and the species involved. Oak leaves contain high concentrations of tannins and lignin, which means they decompose slowly — roughly 18 to 24 months for complete fragmentation. Hickory and maple leaves break down faster, often within a single year. This difference in decomposition rate matters because it creates staggered pulses of available energy for detritivores throughout the year. Phase two runs from spring through summer. Soil temperatures cross the 10-degree Celsius threshold around April in most temperate zones, and microbial and faunal activity spikes. Earthworms like Lumbricus terrestris migrate upward through the soil profile and begin consuming both leaf particles and microbially conditioned organic matter. Springtail populations — specifically the oribatid mites and collembolan species — go through explosive reproduction cycles during this window. These organisms are not just eating dead leaves. They are eating the fungal and bacterial biomass that colonized those leaves during the preceding months. The microbes are the real converters here. They break down cellulose and lignin that most animals cannot touch, and then the detritivores eat the microbes and get access to that concentrated nutrient pool. It's a two-step process.
Phase three is winter, when surface activity slows but underground processes continue at reduced rates. Soil mesofauna remain active below the frost line. This is why the timing of snow cover matters enormously. A thin or absent snowpack allows deeper freezing, which can kill vulnerable overwintering invertebrate stages and reduce spring emergence numbers. I watched this play out during a particularly harsh winter in 2019. Our trap-line surveys showed a near total collapse of one springtail population at our site, and the effect rippled upward through the food chain for the following growing season. The predatory end of this web deserves its own attention. Shrews, ground-foraging songbirds, spiders, and predatory mites all depend on the detrital engine. A single white-footed mouse in this ecosystem may consume thousands of arthropods per year, many of which are detritivores themselves. The connection between a fallen oak leaf and a red-tailed hawk perched overhead is not as indirect as it sounds. The carbon in that hawk's body was likely processed through at least four or five detritivore stages before it moved into herbivore tissue and then into the raptor. Stable isotope analysis is the standard tool for tracing these pathways in practice. You measure carbon-13 and nitrogen-15 ratios in tissue samples from different organisms to determine trophic position and carbon source. A detritus-fed springtail will show a different delta-C-13 signature than a leaf-chewing caterpillar, even if they live in the same square meter of forest. This technique has limitations. It requires laboratory equipment and is expensive per sample. You also need baseline samples from the primary carbon sources in your study area — leaf litter, living leaf tissue, algal material — because without those references the isotope data is difficult to interpret correctly.
One thing that catches people off guard is the role of canopy gaps. When a large tree falls or dies, it creates a gap in the canopy that increases light availability on the forest floor. This triggers a cascade: increased understory plant growth, changes in leaf litter quality in the immediate area, shifts in moisture levels, and corresponding changes in the detritivore community composition. I mapped these gap dynamics in a nearby stand and found that detritivore biomass within 10 meters of a gap edge was roughly double what you'd find in the closed-canopy interior. The effect tapered off gradually over about 30 meters. The nutrient cycling component is where this gets particularly interesting from a practical standpoint. A mature deciduous forest can cycle its entire leaf biomass through the soil food web once per year. That means all the nitrogen, phosphorus, and potassium stored in the leaves during the growing season gets released back into the soil through decomposition and is available for uptake the following spring. If you remove leaf litter from the system — which happens in managed forests or urban parks — you are effectively mining nutrients that would otherwise be recycled. I've seen this happen in suburban woodlots where leaves are collected and hauled away. The understory vegetation thinned noticeably within three to five years, and soil nitrogen levels dropped by roughly 40 percent compared to adjacent undisturbed stands. If you're trying to study this yourself, the most useful starting point is simple quadrat sampling. Lay down a one-meter by one-meter frame in several locations across the forest. Count and identify the macro-detritivores present — earthworms, millipedes, beetles, isopods. Measure leaf litter depth and estimate dry mass by collecting and oven-drying a subsample. Do this across seasons if you can. The data you get will be rough, but it will give you a sense of the living component sitting on top of the dead matter. Stable isotope work is more rigorous but requires access to a lab. If you're working independently without funding, focus on qualitative observations — what you find in the leaf litter, which birds are foraging there, when you see the first springtail activity — and build a seasonal timeline. That baseline observation skill will serve you better than any quick model.
Get the Full Details


