The Motor In The Microbe
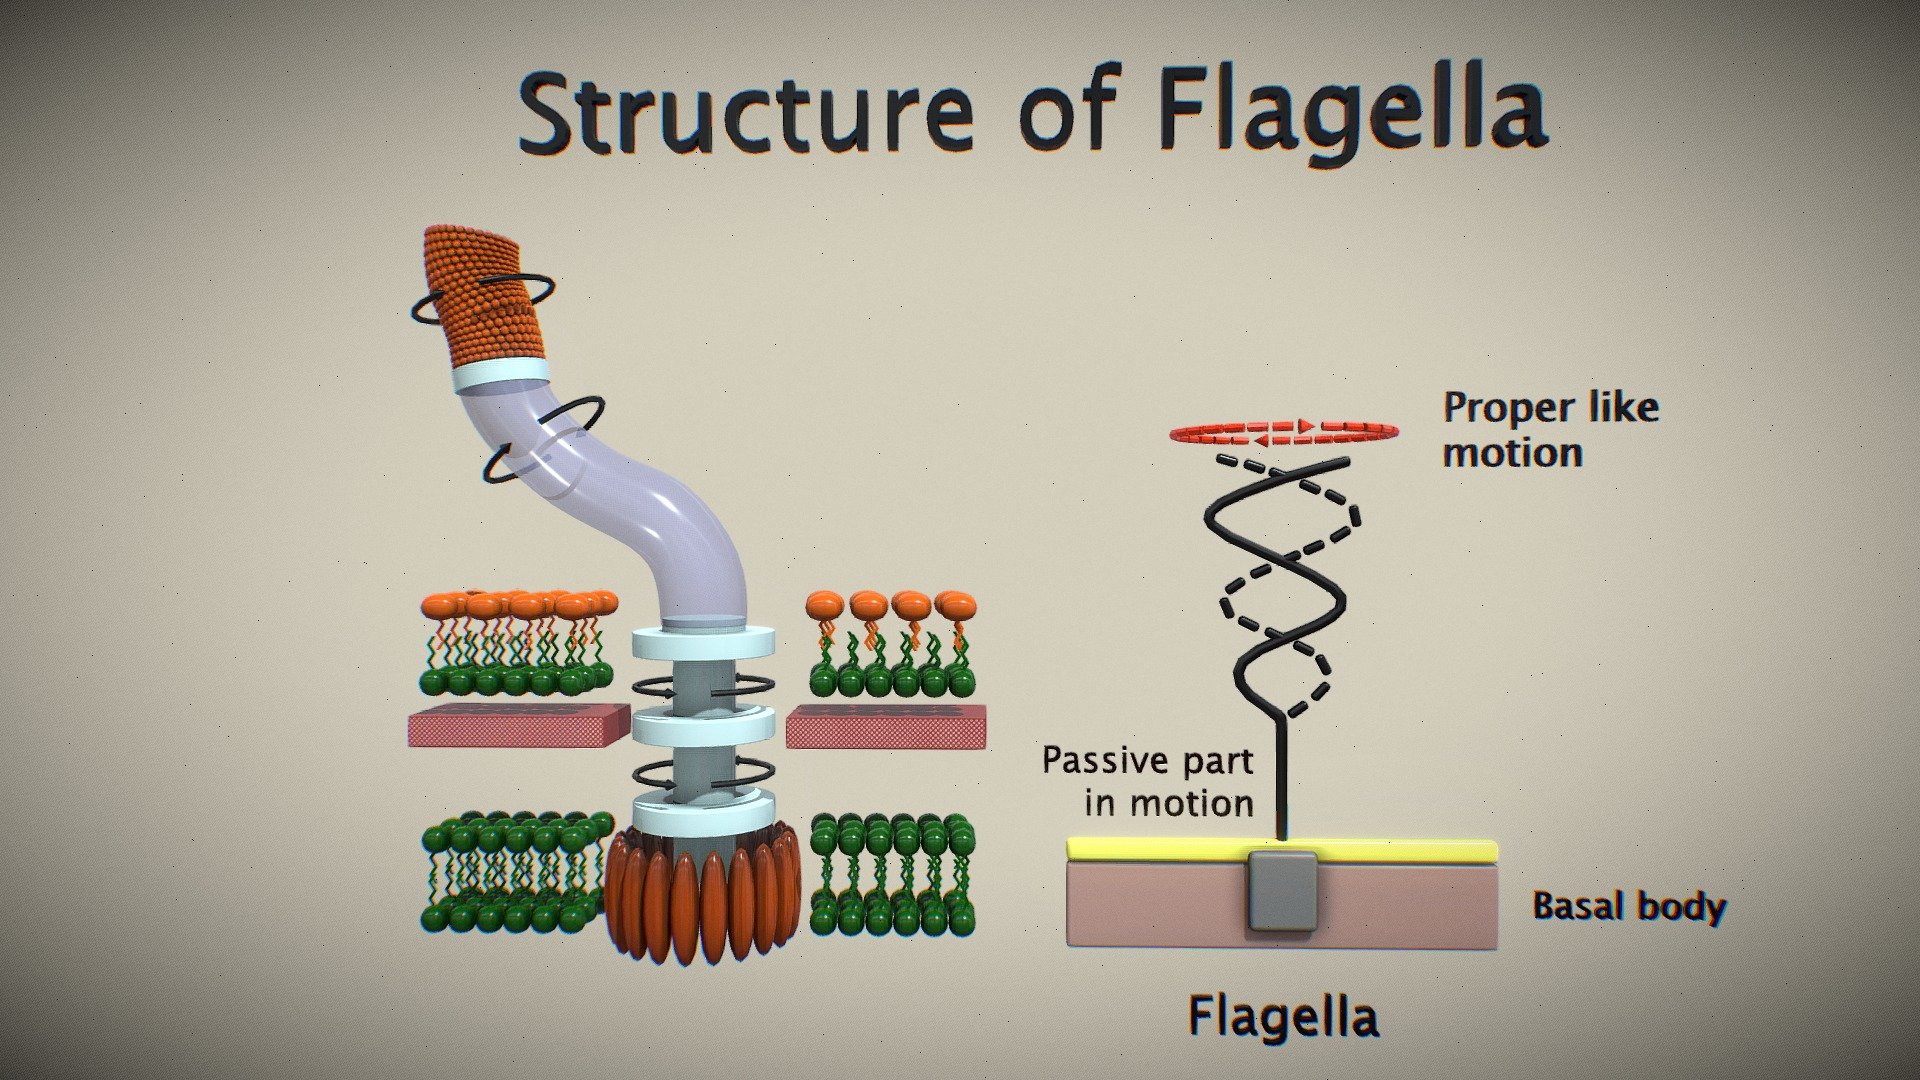
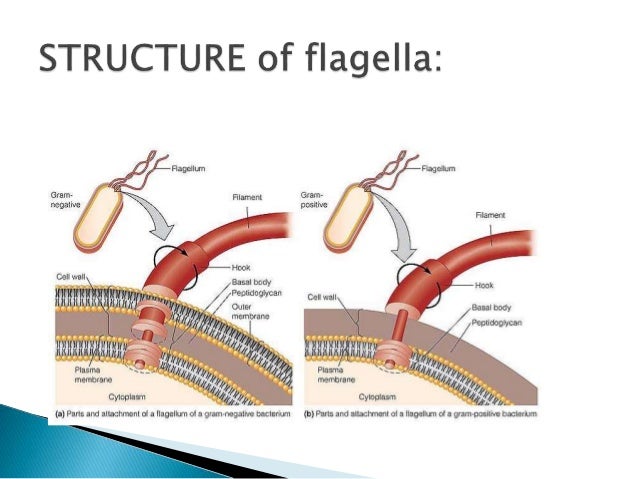
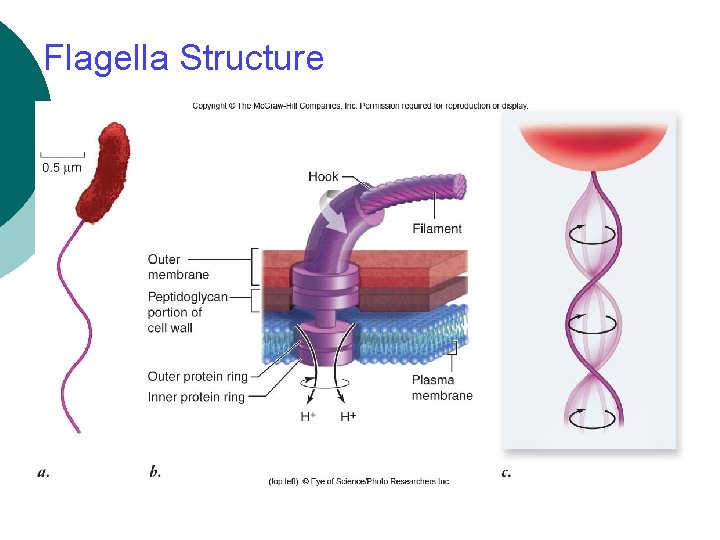
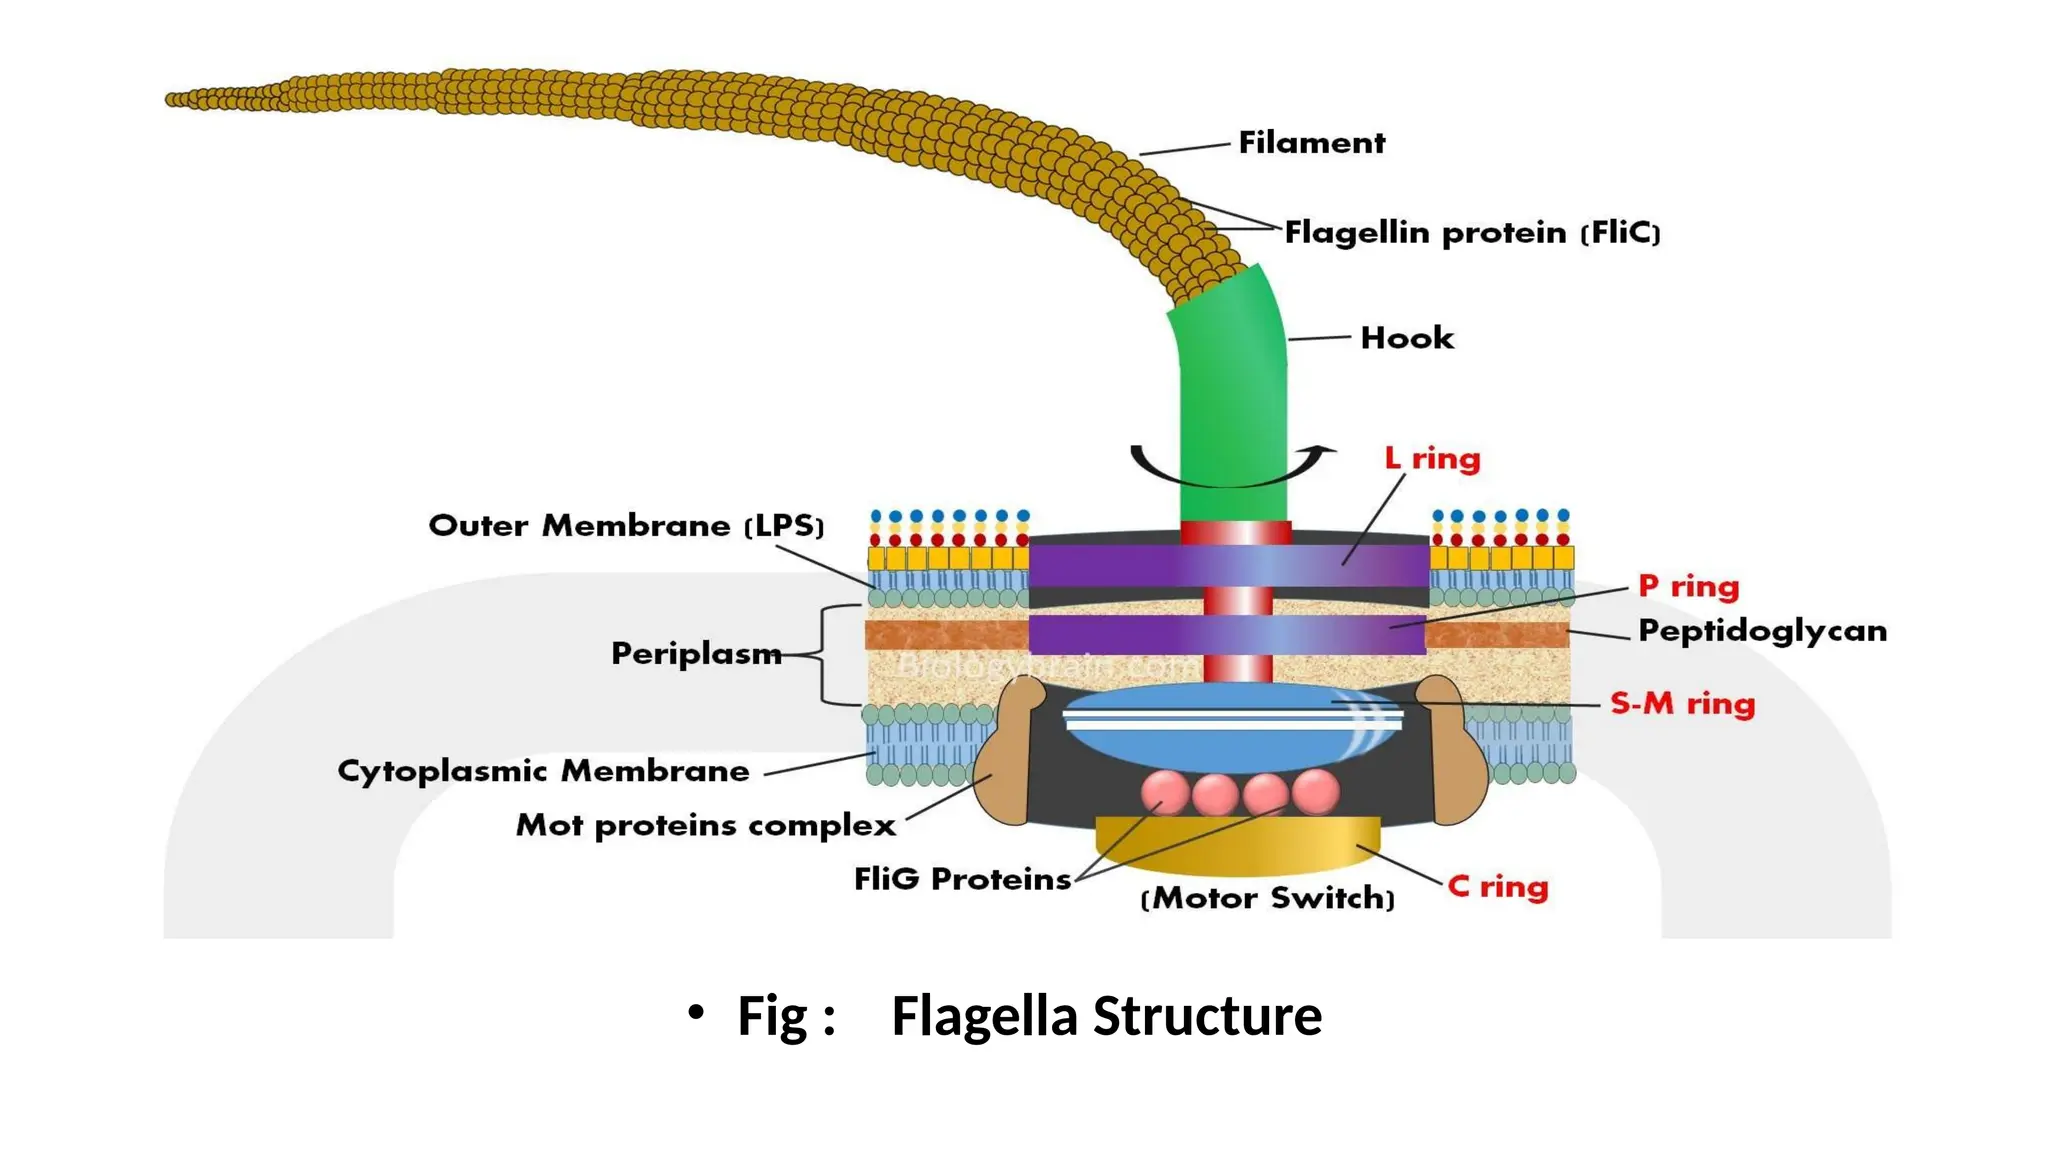
Most people picture a spiral tail and assume it's just a simple propeller. That assumption gets you into trouble fast. Bacterial flagella are among the most complex nanomachines on the planet, and understanding them requires actually looking at how they're built, not just reading a diagram in a textbook. The thing that trips people up when they first start digging into flagellar biology is that the structure isn't what you'd call intuitive. It's a rotary motor embedded in the cell envelope, powered by proton gradients, and it spins at up to 1,000 revolutions per second in some species. I spent about three years working with Salmonella flagellar gene regulation in grad school. Let me tell you where things get messy. The first time I tried to interpret a knockout phenotype, I assumed a single gene deletion would give a clean loss-of-motility readout. It didn't. The flagellar system has cascading regulation — Class 1 genes activate Class 2, which activate Class 3 — and knocking out an early regulator shuts down half the operon without you immediately realizing why. I wasted two weeks chasing what turned out to be polar effects before I re-read the original Nealson and Hastings paper on the hierarchy. Lesson one: read the regulatory cascade before you design the experiment. Here's how the thing actually works under the hood. The basal body sits in the cell envelope and consists of a rod that passes through a series of rings. In Gram-negative bacteria, you've got the M ring embedded in the cytoplasmic membrane, the S ring just behind it in the peptidoglycan layer, then the P ring in the peptidoglycan, and the L ring in the lipopolysaccharide layer. Each ring is made from different proteins. FlgB, FlgC, and FlgF form the rod and the inner rings. FlgG and FlgH make the P and L rings respectively. This whole assembly acts as the rotary bearing. Without it, nothing spins. I remember the moment I actually saw motility recover after complementing a flgC mutant — swimming assays clear within an hour, it's not subtle, and it hits different seeing biology behave exactly as predicted after going through the hassle of the rescue.
The rotor itself is the MS ring plus the C ring, made from FliF and FliG, FliM, and FliN. This is where the switching happens. When the motor rotates counterclockwise, the C ring causes the filament to bundle together and the cell tumbles smoothly forward. Clockwise rotation breaks the bundle and the cell tumbles in place. The switch is controlled by CheY-P binding to FliM in the C ring. It's elegant, but the kinetics are finicky. Getting clean behavioral data requires precise chemotaxis assays, and the stuff falls apart if your agar concentration varies by even one percent. Standardize your media every single time. Now, the filament — that's the propeller part everyone focuses on. It's made of thousands of copies of flagellin (FlaB in many species) polymerized into a hollow tube. The amazing thing is self-assembly. Flagellin subunits travel up through the hollow core of the growing filament and exit at the tip, where they spontaneously incorporate into the structure. No chaperone handed off at the distal end, no ATP hydrolysis at the filament tip. The energy for assembly comes from the binding interactions between subunits themselves. I once tried expressing a fluorescently tagged flagellin in E. coli and watched real-time filament growth using total internal reflection fluorescence microscopy. The tip label showed continuous growth while the base remained dark. Pure polymerization from the end. It took me about six months to get the imaging setup stable enough to capture that, mostly because the signal-to-noise ratio on single-molecule tracking in live bacteria is brutally unforgiving. There's a common misconception that the flagellar motor runs on ATP. It doesn't. It runs on ion motive force — protons in most organisms, sodium ions in Vibrio and a few others. The stator units, MotA and MotB, span the membrane and conduct ions across it. Each ion that flows through creates a conformational change that pushes against the rotor. It's effectively an ion turbine. The torque generated is remarkably constant across different speeds, which is unusual for biological motors. That constant-torque property means the motor can maintain rotation even against increasing viscous load, which matters a lot when you're micrometers long moving through water that feels like molasses at that scale.
One thing nobody warns you about when you're learning this stuff: the export apparatus. The type III secretion system at the base of the flagellum is responsible for pumping flagellar proteins out of the cytoplasm and through the narrow central channel of the growing filament. This is a dedicated protein export machine, and it's thermodynamically uphill. It uses the same ion gradient that powers the motor, coupled through structural components of the basal body. I spent a chunk of my postdoc characterizing point mutations in the export gate protein FleQ and learned the hard way that even single amino acid changes in the selector plug can completely block substrate specificity. You think you're studying export, and suddenly you've accidentally rewired the entire recognition hierarchy for which proteins get exported at which phase. Not fun to debug. Regulatory complexity is another area where beginners get burned. The flagellar gene network in enteric bacteria involves roughly 50 genes organized into three transcriptional classes. Class 1 encodes the master regulator FlhD4C2, which activates Class 2 promoters. Class 2 includes FliA, the sigma factor for Class 3 genes, but FliA is sequestered by the anti-sigma factor FlgM. Here's the catch: FlgM is only exported after the hook-basal body is complete, which means the cell waits until the motor scaffold is built before committing resources to the filament and the chemotaxis machinery. This checkpoint is non-negotiable. Mutants that can't degrade FlgM constitutively never express Class 3 genes and remain non-motile regardless of anything else you throw at them. I learned this when a colleague's strain looked completely WT except it never expressed the filament, and we tore the whole plasmid map apart looking for a mutation before someone remembered to check FlgM levels by western blot. The chemotaxis response itself is another layer of complexity. It's not just on-off switching of the motor. It's a perfect-adaptation system involving methylation of methyl-accepting chemotaxis proteins (MCPs) by CheR, and demethylation by CheB. This feedback loop allows the cell to reset its sensitivity after a stimulus, so it can keep sensing gradients indefinitely. The kinetics here are fast — adaptation happens on the order of seconds. But the system is sensitive to temperature, ionic strength, and even the growth phase of the culture. Running chemotaxis assays with overnight cultures gives different results than assaying mid-log phase cells. Always report your growth conditions. People skip that and then wonder why their tumble bias numbers don't match the literature.
Get the Full Details
If you're working with flagella experimentally, one practical note: isolating intact flagellar filaments is harder than it sounds. Standard lysis buffers shear the filaments unless you keep everything cold and add protease inhibitors. I use a gentle sonication protocol on ice, followed by low-speed centrifugation to remove whole cells and debris, then ultracentrifugation at 100,000 times g for two hours to pellet the filaments. The resulting pellet is nearly pure flagellin, but you'll need to verify integrity by SDS-PAGE — degraded filaments show smearing instead of a sharp band at around 50 to 55 kilodaltons depending on the organism. Native flagellin runs differently, too. If you're doing structural work, crosslinking before lysis can help preserve the supramolecular architecture. The evolutionary angle is also worth noting because it keeps coming up in papers. The flagellar type III secretion system shares homology with the needle complexes of pathogenic bacteria like Yersinia and Pseudomonas. This isn't speculation — structural studies show near-identical folding in the export apparatus components. Some researchers argue this means the flagellum evolved from a secretory system, others say they share a common ancestor. Both positions have merit. What's not debatable is that the genetic toolkit for building a flagellum is conserved across vast evolutionary distances, and horizontal gene transfer has moved flagellar genes between species in ways that complicate phylogenetic reconstruction. If you're using flagellar genes for bacterial typing or phylogeny, be aware that the tree you get might reflect the history of the gene, not the organism. For anyone starting out, I'd recommend picking a single well-characterized model — E. coli or Salmonella enterica — and reading the original papers rather than relying on review articles. The reviews smooth over the uncertainties. The primary literature shows you where the disagreements are. Start with the Macnab and Williams paper on the flagellar assembly hierarchy, then move to the later work by Hughes and Kutsuna on the export apparatus, and don't skip the older biophysical papers from Berg and colleagues on motor torque. Those experiments were done with optical tweezers attached to individual cells, and they established the fundamental properties of the motor that still hold today. Sometimes the old data is better than the new reviews.
I should mention one failure mode that catches people off guard. Not all bacteria use proton-driven motors. Some species, notably the marine Vibrios, use sodium ions. The stator units in those organisms are MotPS or Na+-specific variants of MotAB, and they won't function in standard E. coli expression systems because the sodium gradient isn't maintained the same way. If you're heterologously expressing a flagellar system, check the ion requirement before you bother with the rest. I've seen grant proposals built around motor mechanics that were doomed from page one because the authors didn't account for this. The flagellum is also a major virulence factor in many pathogens. It's recognized by Toll-like receptor 5 in humans, and the immune response to flagellin is significant. This has practical implications if you're doing any kind of immunology work — contaminated cultures can trigger inflammation in your assays, and flagellin is one of the most immunogenic bacterial proteins known. I had a cell culture experiment fail because a colleague's flagellated strain contaminated a culture, and the TLR5 response in our human cell line skewed the cytokine readout by orders of magnitude. Screen for motility, plate on non-motility-selective media if you're working with immune cells. Just something to keep in mind. There's been a lot of excitement recently about artificial flagellar motors and synthetic nanomachines inspired by biology. The physics of what natural flagella do at low Reynolds number doesn't translate well to macroscopic analogs. A screw-shaped propeller that works at biological scale generates almost no thrust when you scale it up because inertia dominates over viscosity. If you're trying to build something inspired by flagellar propulsion, you need to think about the actual biophysical constraints, not just the geometry. The spiral shape matters because of how it interacts with a viscous fluid, not because it looks like a propeller. That's a distinction that gets lost in a lot of the popular science coverage.
The basic toolkit for studying flagella hasn't changed dramatically in twenty years — swimming assays, swarm plates, electron microscopy, genetics. But the tools you can layer on top of that have. Cryo-EM has resolved the flagellar motor at near-atomic resolution in the past decade, showing you exactly how the stator units engage with the rotor. Single-molecule fluorescence lets you track individual flagellin subunits as they're exported. Microfluidics gives you controlled chemical gradients at the scale of individual cells. These techniques are making it possible to ask questions that were impossible ten years ago. The field is moving fast, but the fundamentals remain the same. Understand the motor, understand the assembly, understand the regulation. Everything else builds on that.