Food Web Modeling From Scratch
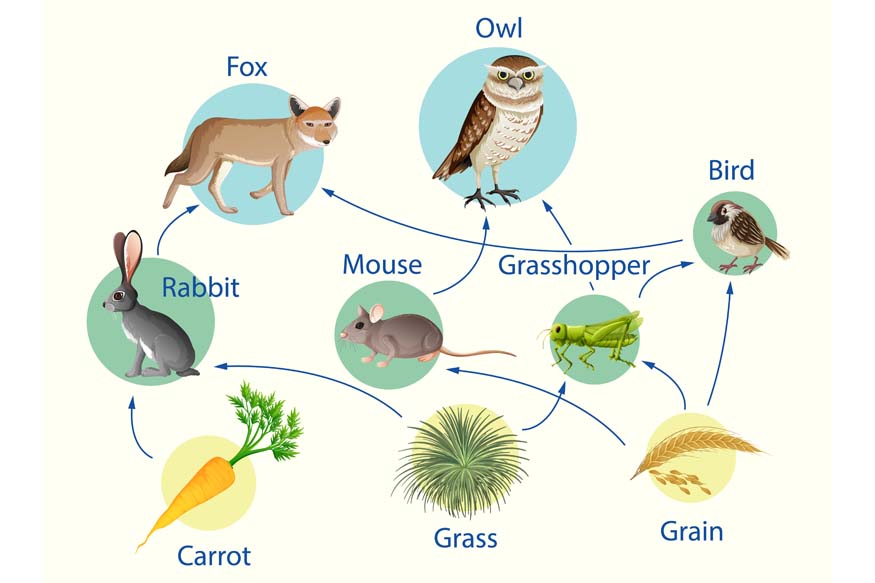
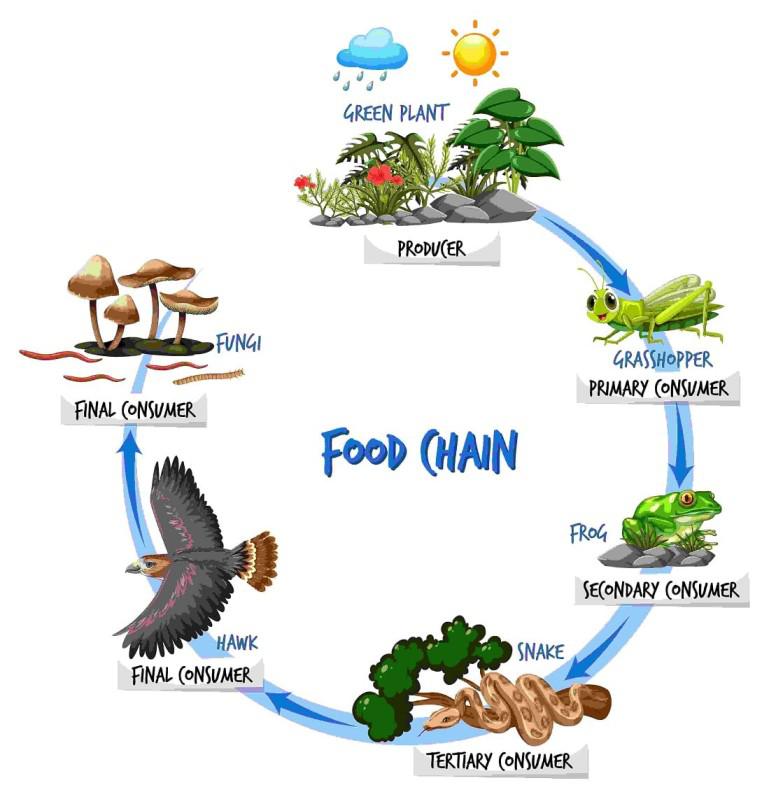
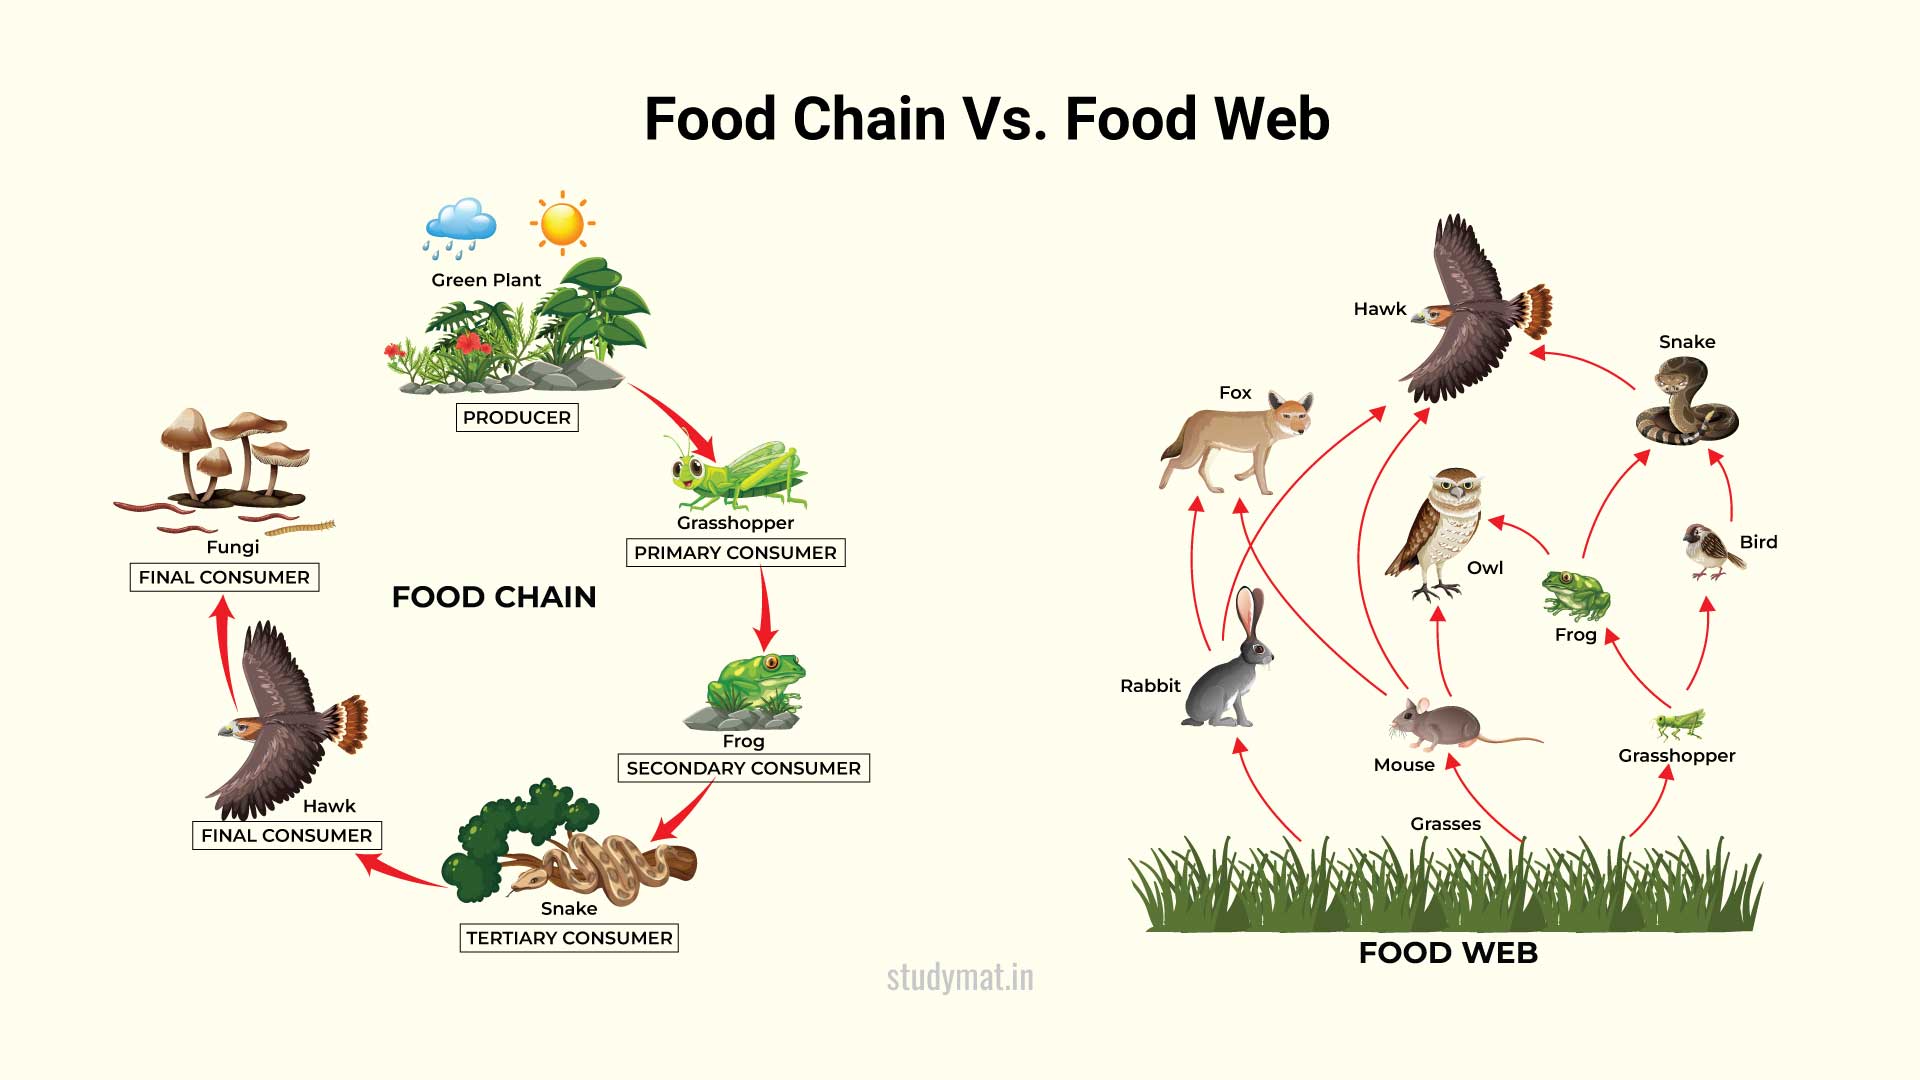
Building a functional food chain model requires tracking trophic levels, energy transfer efficiency, and species interaction strength across multiple layers. Most people treat this as a simple top-down hierarchy where producers feed primary consumers who feed secondary consumers, but that oversimplification breaks down the moment you introduce omnivory, detritivores, or seasonal migration patterns into the system. The first step is mapping your system boundaries. Are you modeling a single pond, a coastal marine zone, or a terrestrial grassland? I once spent three weeks building a food web for a temperate forest micro-habitat only to realize I had completely ignored the fungal network and soil mesofauna that process roughly forty percent of the primary productivity. That oversight skewed every energy flow calculation downstream. The fix was to pull leaf litter sampling data from the local university extension office and build a separate detrital pathway that ran parallel to the grazing chain. Trophic level assignment comes next, but it is not as straightforward as labeling every organism. Many species shift trophic positions depending on life stage, season, and prey availability. A juvenile fish might sit at trophic level 2.1 while the same species as an adult feeds predominantly on other fish and rises to level 3.8. Use stable isotope analysis data when you can get it. If you are working from literature values alone, assign each consumer a fractional trophic position based on stomach content surveys rather than rounding to whole numbers.
Energy transfer between trophic levels follows the ten percent rule on average, but that figure is a rough heuristic, not a law. Actual transfer efficiency ranges from about five to twenty percent depending on organism type, temperature, and ecosystem productivity. Cold-blooded predators in nutrient-poor systems often show transfer efficiencies closer to eight percent, while warm-water planktonic chains can hit fifteen or sixteen percent. Your model will produce wildly different biomass pyramids if you assume a flat ten percent across all transitions.
Building The Interaction Matrix
An interaction matrix is the backbone of any food web model. Each row represents a species, each column represents a potential prey or resource, and the cell values describe the strength of the connection. The values can be binary or weighted by consumption rate, biomass proportion, or encounter frequency. Weighted matrices give you something closer to reality but they demand data you may not have. I recommend starting with presence-absence data from published food web databases like Web of Life or GloBI, then layering in local diet studies to adjust connection strengths. A common mistake is treating all links as equally strong. In practice, a predator might consume fifteen prey species, but eighty percent of its energy comes from three of them. Weight those dominant links at 0.6 to 0.8 relative strength and the weak links at 0.05 to 0.15. Connectance, the ratio of observed links to possible links, is a useful descriptor. Most real ecosystems fall between 0.05 and 0.3 connectance. If your model outputs a connectance above 0.4 for a complex habitat, you likely overestimated niche overlap or included omnivorous feeding links that do not actually occur at meaningful rates. If it drops below 0.03, you probably missed key mutualistic or opportunistic interactions.
Get the Full Details
Dynamic Simulation Steps
Once your matrix is built, you can run a basic Lotka-Volterra consumer-resource simulation or a more structured niche model. Start simple. Use differential equations where the growth rate of each species depends on resource availability and predation pressure. The classic formulation looks like this for a consumer population: dN_i/dt = N_i * (sum of e_j * a_ij * N_j - sum of a_ik * N_k - m_i) Where N is population, e is conversion efficiency, a is attack rate, and m is mortality. Running this with realistic parameter values will show you how stable or volatile your system is. I found that small changes in top predator mortality rates, less than five percent, can cascade into complete regime shifts within fifty to eighty simulation years in my grassland model. The system flipped from a herbivore-dominated state to an algal-bloom state when I adjusted the predator parameter slightly.
Bifurcation analysis is worth doing if you want to identify tipping points. Sweep one parameter across a range while holding others constant and plot equilibrium biomass for each species. The points where curves fold back on themselves mark critical thresholds. This is where food chain theory meets practical conservation. Knowing that a fourteen percent reduction in tertiary consumer biomass triggers a trophic cascade saves more effort than trying to manage the system after the collapse.
Pitfalls And Where The Approach Fails
Static food web models, which is what most people build first, cannot capture seasonal dynamics, phenological mismatches, or behavioral plasticity. A model run once with averaged parameters will look elegant and tell you almost nothing about what happens when spring floods alter prey accessibility or when a disease event removes a keystone species mid-season. Dynamic models that incorporate time-varying parameters solve this partially but require parameter sets you often cannot source from published literature. Another limitation is the assumption of mass balance closure. Real ecosystems exchange energy and organisms across boundaries through immigration, emigration, and atmospheric deposition. If your study area is an isolated wetland with no hydrological connections, the assumption holds better. For riparian or marine systems, boundary fluxes can account for thirty to sixty percent of total energy input, and ignoring them makes your model systematically underestimate carrying capacity for intermediate consumers. The practical workaround I use is to add a fuzzy boundary layer. Treat unspecified immigration and emigration as a noise term added to the equations for migratory species, and run Monte Carlo simulations with that term drawn from a uniform distribution between negative and positive values proportional to the estimated boundary flux. It does not give precise predictions but it gives you confidence intervals that actually reflect uncertainty rather than false precision.

Interpreting Model Output
After running your simulation, look at three metrics: total system throughput,ascendancy, and omnivory index. Total system throughput measures the total flow of energy through the web per unit time and tells you whether your model is producing biologically reasonable productivity values. Ascendancy, which combines throughput with information flow structure, indicates how organized and efficient the energy routing is. A high ascendancy relative to capacity means the system has evolved strong preferential pathways rather than distributing energy randomly. The omnivory index captures the fraction of links that connect species more than one trophic level apart, which is a proxy for food web complexity and stability in most theoretical frameworks. If your output shows an omnivory index above 0.6 in a simulated system, question your link assignments. Most natural food webs sit between 0.15 and 0.45. Values above 0.6 usually indicate that you have double-counted links or incorrectly assigned predators to resources they do not actually consume at meaningful rates. Review the matrix cell by cell and cross-check against primary literature for each questionable connection. Sensitivity analysis is non-negotiable before you publish or present any model result. Perturb each parameter individually by ten percent and record the change in equilibrium biomass for every species. Parameters that cause large biomass shifts are your controlling factors. In my forest micro-habitat model, decomposer efficiency had more influence on primary producer biomass than any consumer parameter, which was not intuitive from a traditional top-down trophic cascade perspective. That finding redirected my entire interpretation of the system.
Food web modeling is a tool for generating testable hypotheses, not a crystal ball. The best models I have built were useful because they revealed which processes mattered most and which assumptions I should discard, not because they predicted exact population trajectories. Treat your results as directional guidance and always validate against field observations when you can.