The Long Wait For Bare Rock
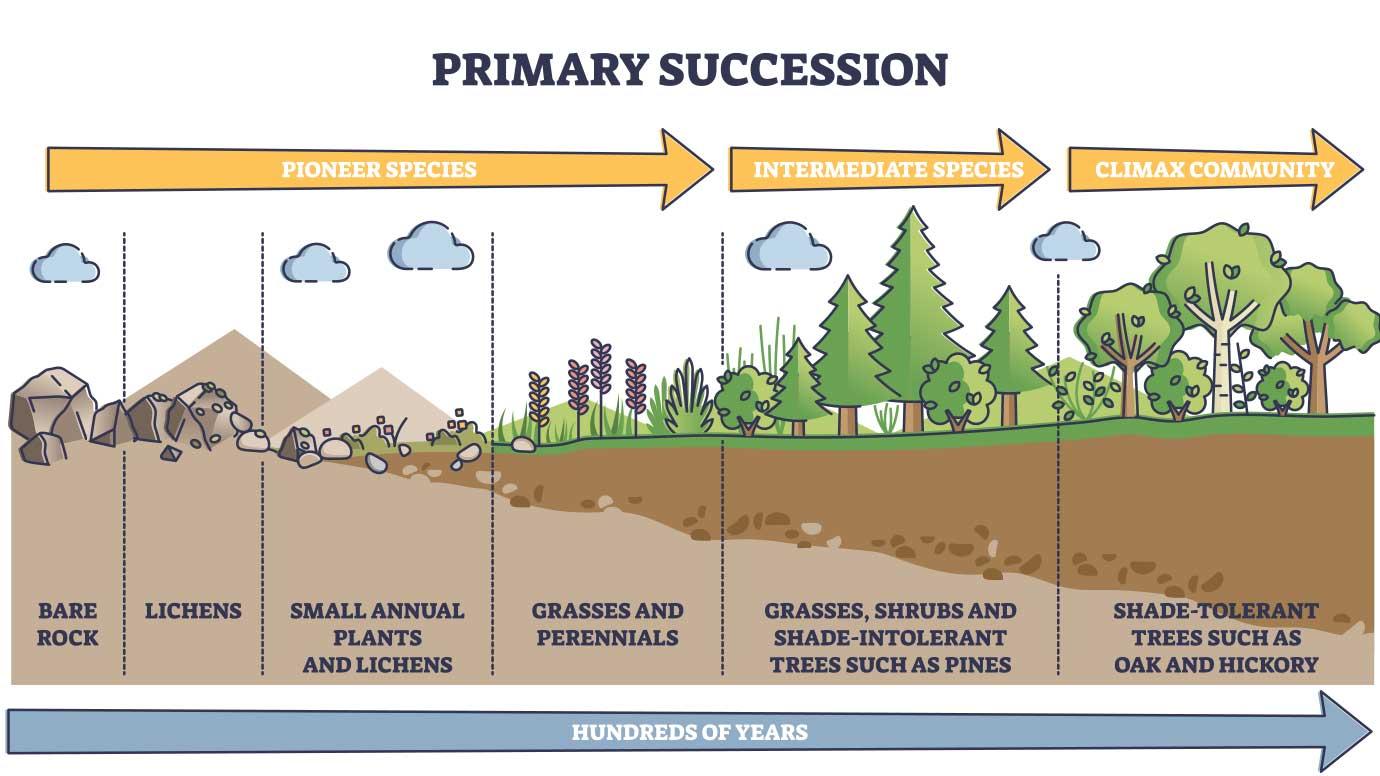
I spent three summers monitoring a lava flow in Iceland where nothing had grown for roughly forty years. The first thing you learn is that primary succession isn't a race. It is agonizingly slow, and most of what you will read in textbooks glosses over how much of it just sits there doing absolutely nothing for decades at a time. When people ask me how to think about ecological restoration on bare substrate, I tell them to start by accepting that the timeline will embarrass you. Primary succession happens when life colonizes a surface that has never supported organisms before. Fresh volcanic rock, retreating glaciers leaving behind till, sand dunes that have baked dry, or mine tailings stripped to the parent material. There is no soil. There is no seed bank. There is nothing but mineral substrate and whatever propagules can reach it by wind, water, or animal transport. That is the starting condition, and the simplicity of it is misleading. The actual process unfolds in phases, though not always in the neat sequence you find in lecture slides. Pioneer organisms arrive first, almost always cyanobacteria, lichens, and mosses. These are not random choices by nature. They are the only things with the physiological toolkit to handle direct UV exposure, desiccation, and the complete absence of nutrients. Lichens secrete organic acids that etch microscopic channels into silicate rock. Over years, that weathering releases trace minerals. When the lichen dies, it leaves behind a crust of organic material. Mosses then root into that crust. Each generation builds a fraction of a millimeter of proto-soil.
I remember standing on that basalt field in Iceland and trying to measure net primary production with a portable photosynthesis system. The reading was essentially zero. Not negative. Just zero. The crustose lichens were metabolically active at a level far too low for the to register. That is the kind of detail fieldwork teaches you that papers omit. The pioneers are working, they are just operating at a scale that is invisible to standard measurement tools. Once you have enough organic matter to hold water, annual plants and herbaceous perennials can establish. Grasses, then legumes if nitrogen-fixers happen to be present in the propagule pool. Shrubs follow. Then trees. The trajectory from bare rock to forest can take anywhere from two hundred to eight hundred years depending on climate, elevation, and proximity to seed sources. That is not a range I am padding for effect. It is the observed spread across subarctic and alpine sites in the Pacific Northwest.
What Actually Determines The Pace
Climate is the obvious factor. Moisture and temperature control weathering rates and decomposer activity. But the less obvious factor is biotic interaction, and this is where beginners consistently get it wrong. They assume each stage simply replaces the previous one through competition. The reality is messier. Facilitation matters enormously in the early phases. Lichens create the conditions that mosses need. Mosses create the conditions grasses need. Without that ladder, the later species cannot reach the site because there is literally nothing to root into. Nitrogen fixation deserves its own emphasis. In many primary succession sequences, the transition from bryophyte dominance to vascular plant dominance hinges on whether a nitrogen-fixing partner has arrived. Cyanobacteria in lichen thalli fix atmospheric nitrogen, but the rates are tiny. When a nitrogen-fixing shrub like Ceanothus or Alnus shows up, the whole system accelerates. Soil nitrogen can increase by an order of magnitude within a single decade. That is the kind of inflection point that determines whether you end up with a fast-growing conifer stand or a stunted scrub community that persists for centuries. Propagation source distance is another constraint nobody wants to hear about but everyone ignores. If your bare substrate is more than fifteen kilometers from a mature forest, woody plant colonization becomes statistically unlikely without human assistance. Wind disperses seeds, yes, but most tree seeds do not travel that far in viable condition. Birds move some, but the dispersal kernel drops off sharply after ten kilometers. This is not theory. I have seen exactly this play out on glacial forefield sites where the nearest tree line was thirty kilometers away and the initial plant community consisted entirely of herbs and grasses with no woody species in sight.
Get the Full Details
Restoration Work On Primary Substrate
If you are attempting restoration on a site that qualifies as primary succession terrain, you are working with broken geomorphology, not broken ecology. The ecosystem was never there to begin with, so you cannot restore it to a prior state. You can only establish conditions that allow the natural sequence to proceed. That distinction matters because it changes every decision you make. Soil creation is the bottleneck. You can accelerate it, but you cannot skip it. The practical approach is to introduce organic matter and microbial inoculum. I have used shredded bark and composted wood fiber spread at roughly four centimeters thick over stabilized substrate. It sounds trivial, but the difference between an untreated plot and an inoculated one becomes visible within two growing seasons. The treated plots develop earthworm activity and fungal hyphal networks much sooner, which increases water retention and nutrient cycling. Seeding strategy requires patience and specificity. Broadcasting wildland seed mix is adequate for secondary succession sites where some soil exists. On primary substrate, you need to target the pioneer species first. Nostoc-infected lichens can be cultivated on sterile pumice and spread directly onto fresh lava. Moss propagules mixed with clay slurry can be hydroseeded onto slopes. These are not elegant solutions. They are labor-intensive and they fail often. But they are the only methods that actually work without importing mature soil, which defeats the purpose of working on a primary site.
Edge Cases And Where Standard Approaches Break
I worked a site once where the parent material was crushed basalt from a quarry, and every restoration protocol we tried failed. Lichen culture died within weeks. Moss slurry washed away in the first rain. Seedlings of native grasses died from aluminum toxicity in the freshly crushed rock. The problem was that the crushing process had fresh, reactive surfaces that released soluble aluminum at concentrations toxic to most plant roots. Standard restoration guides do not cover this because it is rare enough that nobody writes papers about it. The workaround was to apply a calcium carbonate amendment at two metric tons per hectare, which neutralized the aluminum availability and raised the pH to a range where pioneer microbes could establish. After six months of microbial colonization, the lichen cultures finally took. It added fourteen months to the project timeline and roughly eighteen thousand dollars in materials, but it was the only intervention that shifted the chemistry enough for biological processes to take over. Without that amendment, nothing else would have worked regardless of how well you executed the biological components. There is also the issue of chronic nutrient limitation that persists long after you think the system should have moved past it. In subarctic environments, phosphorus often becomes the limiting nutrient after nitrogen is no longer scarce. I have monitored sites where legume-dominated patches saturated the soil with nitrogen but stunted growth because the underlying basalt simply does not weather fast enough to release phosphorus. Adding phosphate fertilizer is an option, but it creates dependency and alters the successional trajectory in ways that make the eventual climax community unreliable. The tradeoff is real and it is rarely discussed in restoration planning documents.
What Primary Succession Models Miss
Connell and Slatyer's three models of succession facilitation, tolerance, and inhibition are useful frameworks but they are too clean for field application. In practice, all three mechanisms operate simultaneously on different patches within the same site. You might see facilitation on the leeward side of a boulder where moisture accumulates and inhibition on the windward side where desiccation kills emerging seedlings before they establish. The model tells you which mechanism dominates, but it does not tell you how to manage a heterogeneous landscape where both are happening at once. Another gap is the assumption that succession is directional and predictable. It is not. Climate fluctuations, disturbance events, and stochastic colonization orders can push a site into alternative stable states. A heath-dominated plateau and a birch-dominated woodland can occupy the same climatic niche on similar substrates. The difference comes down to which species arrived first and whether they modified the environment in a way that excluded the other. Once that path is set, reversing it requires active intervention, not just waiting. The bigger limitation is that primary succession models assume sufficient time between disturbances for the sequence to progress. In landscapes subject to frequent volcanic activity, glacial advance, or industrial disturbance, the system may never reach a late-successional stage before it gets reset. Restoration practitioners in those environments need to abandon the goal of reaching a climax community and focus on maintaining functional ecosystem processes instead. That means prioritizing nutrient cycling, water retention, and habitat connectivity over species composition targets that may be ecologically unreachable.
Practical Monitoring Metrics That Actually Matter
Most restoration projects track plant species richness and cover percentage. Those metrics are fine for secondary succession but nearly useless for primary succession because the early community will always look depauperate regardless of whether the process is proceeding correctly. Instead, measure soil organic carbon, water infiltration rate, and microbial biomass carbon. These three indicators respond to biological activity before visible plant changes occur. A rise in microbial biomass typically precedes the first vascular plant emergence by one to two growing seasons. Infiltration rate is especially informative. Fresh basalt and glacial till have high infiltration when dry but can develop surface crusting that reduces infiltration once biological activity begins. A temporary decrease in infiltration followed by a recovery is actually a positive sign. It means crusts are forming, which stabilizes the substrate and creates microhabitats. If infiltration keeps increasing linearly without that dip, the crust is not developing properly and the site is likely losing material to erosion rather than building soil. I track crustose lichen coverage using a point-intercept frame at fixed stations. It takes about twenty minutes per site and gives me data I can compare year to year. Percentage cover in the first five years is usually below five percent. When it crosses ten percent, I know the system is transitioning out of the earliest phase and nutrient accumulation is beginning to accelerate. Below that threshold, any intervention you make is fighting an uphill battle against the fundamental constraints of the substrate. Above that threshold, biological momentum is building and interventions become much more effective.
When To Walk Away
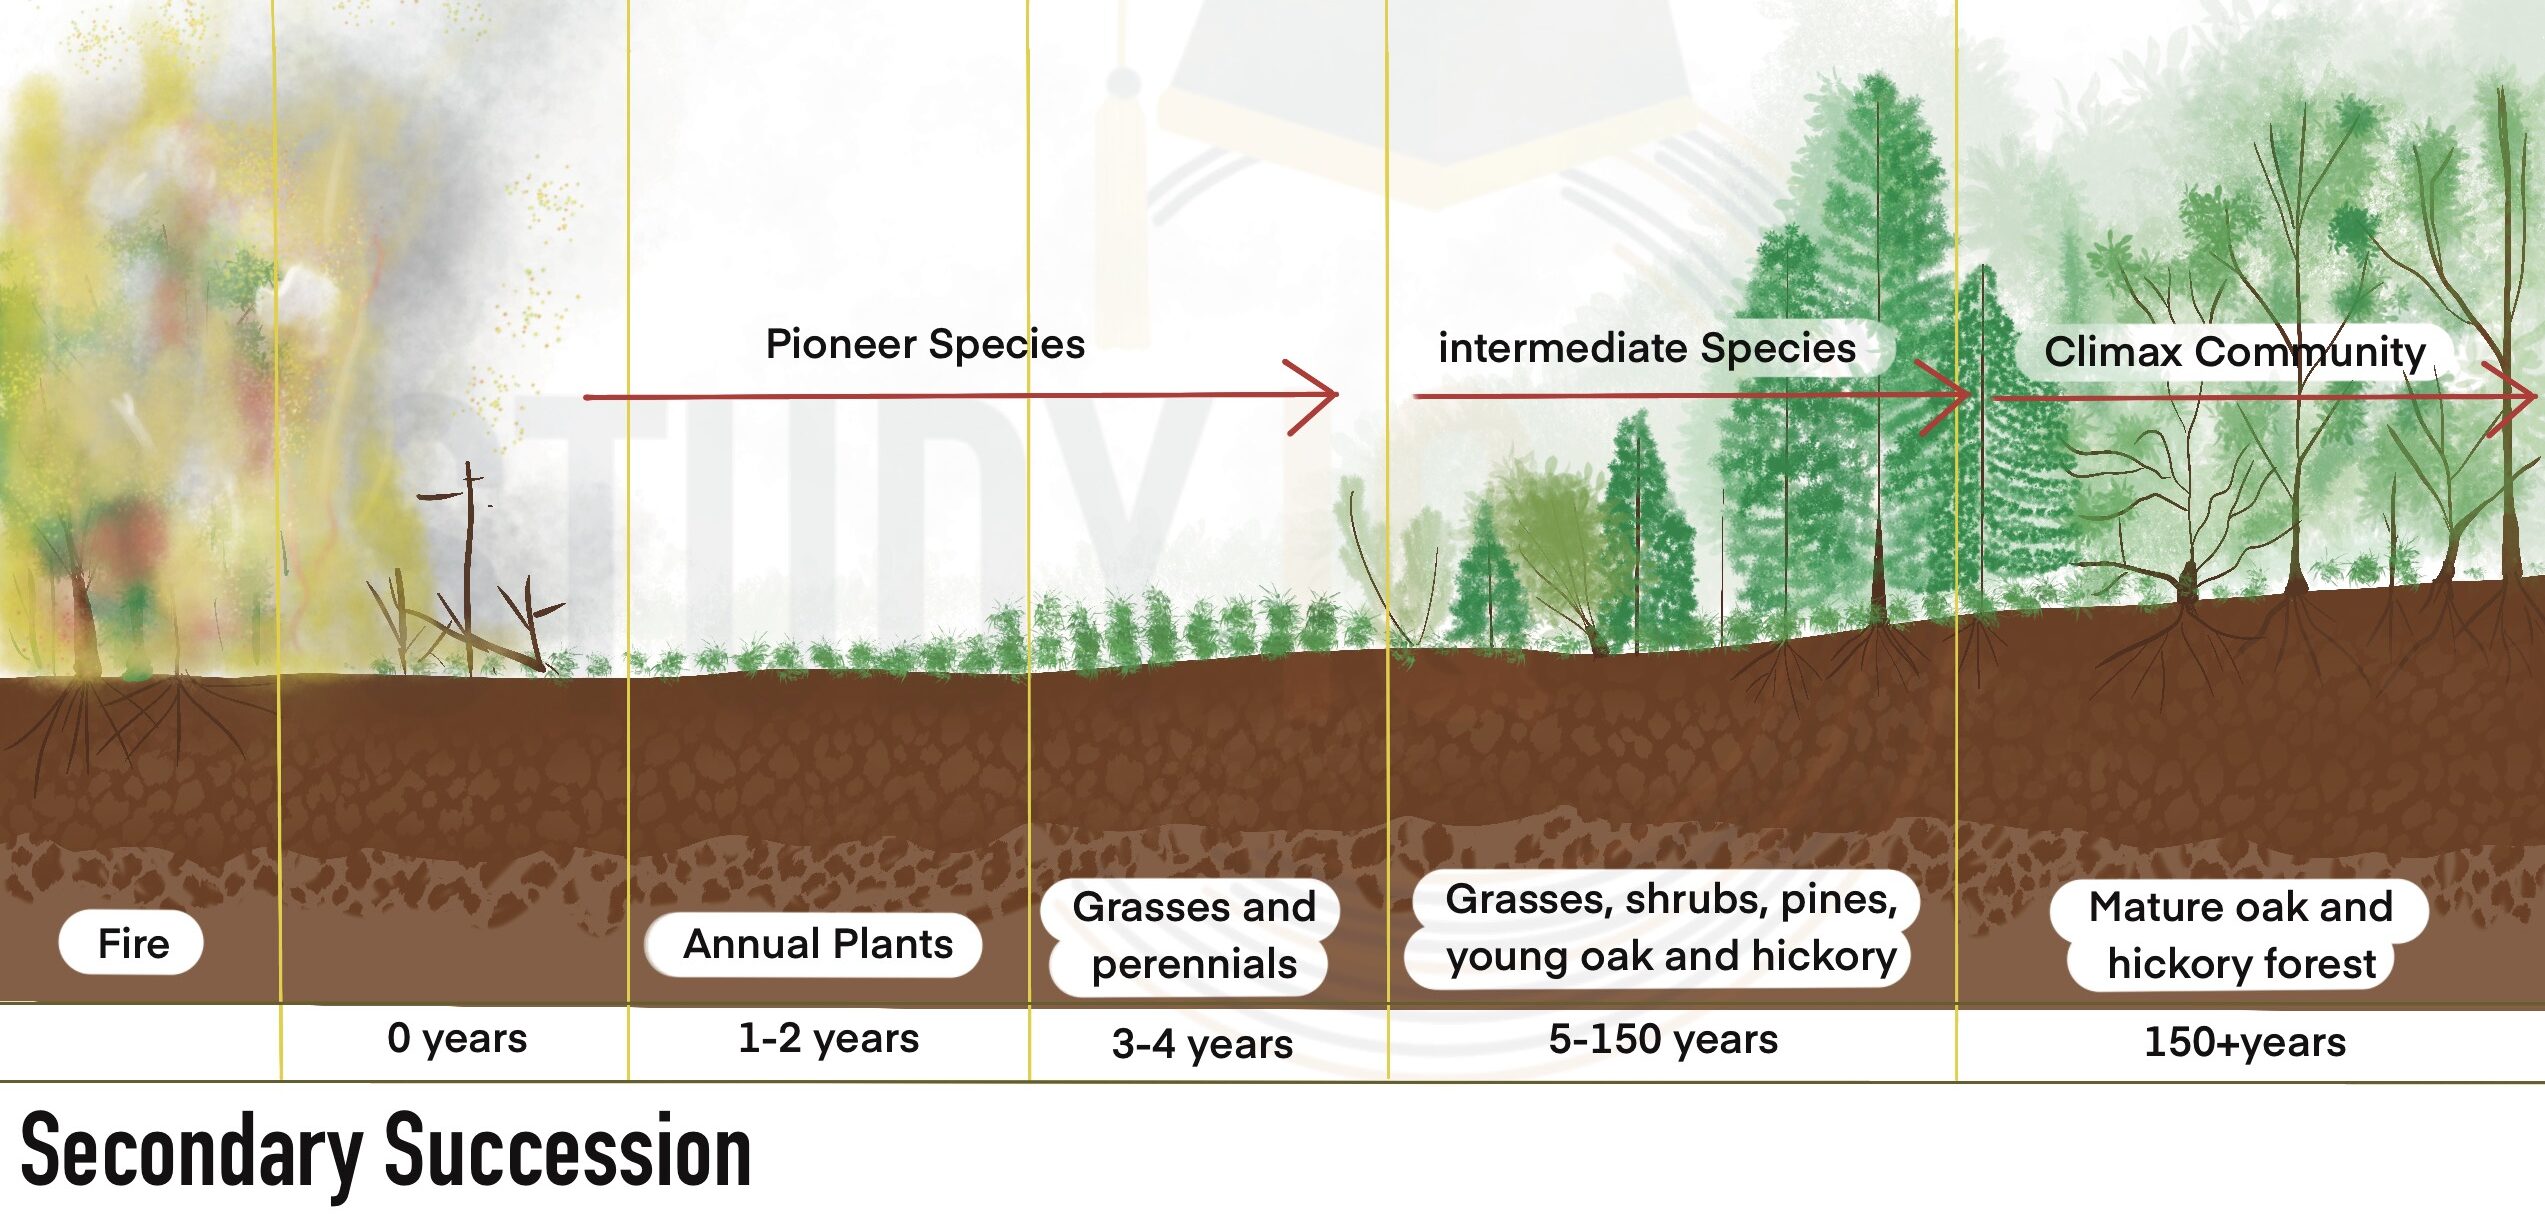
Primary succession restoration has a threshold beyond which intervention becomes economically irrational. If the substrate is highly weathered rock with some soil development already occurring, waiting is often the best strategy. Nature will recolonize it given enough time and propagule availability. Active restoration makes sense when the substrate is fresh, sterile, and exposed to erosion, or when the site is within a restored landscape matrix that requires ecological connectivity to function. It does not make sense on large tracts of isolated barren ground where the cost of soil amendment and species introduction exceeds the ecological value of the intervention by a wide margin. The sites where active restoration fails most often are those where the practitioner has confused primary with secondary succession. Applying topsoil, mulch, and fast-growing cover crops to a site that should be left to pioneer colonization introduces nutrients and species that short-circuit the natural sequence. The result is a weedy, nutrient-dependent community that collapses once the imported materials degrade. The site ends up with less biodiversity and worse soil structure than it would have developed on its own. This happens more frequently than I would like to admit in the restoration industry. Primary succession is not a problem to solve. It is a process to observe and occasionally assist. The assistants who last are the ones who understand when their presence matters and when it does not. The rest is just geology waiting for biology to catch up.