Understanding Primary Consumers in Ecosystems
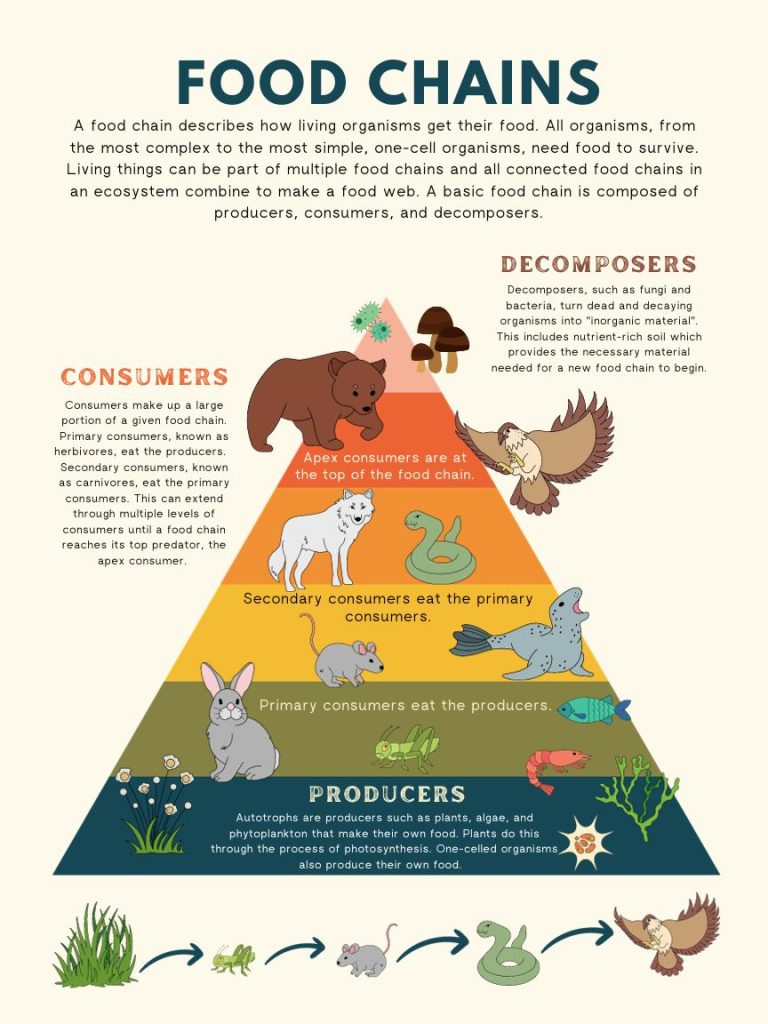
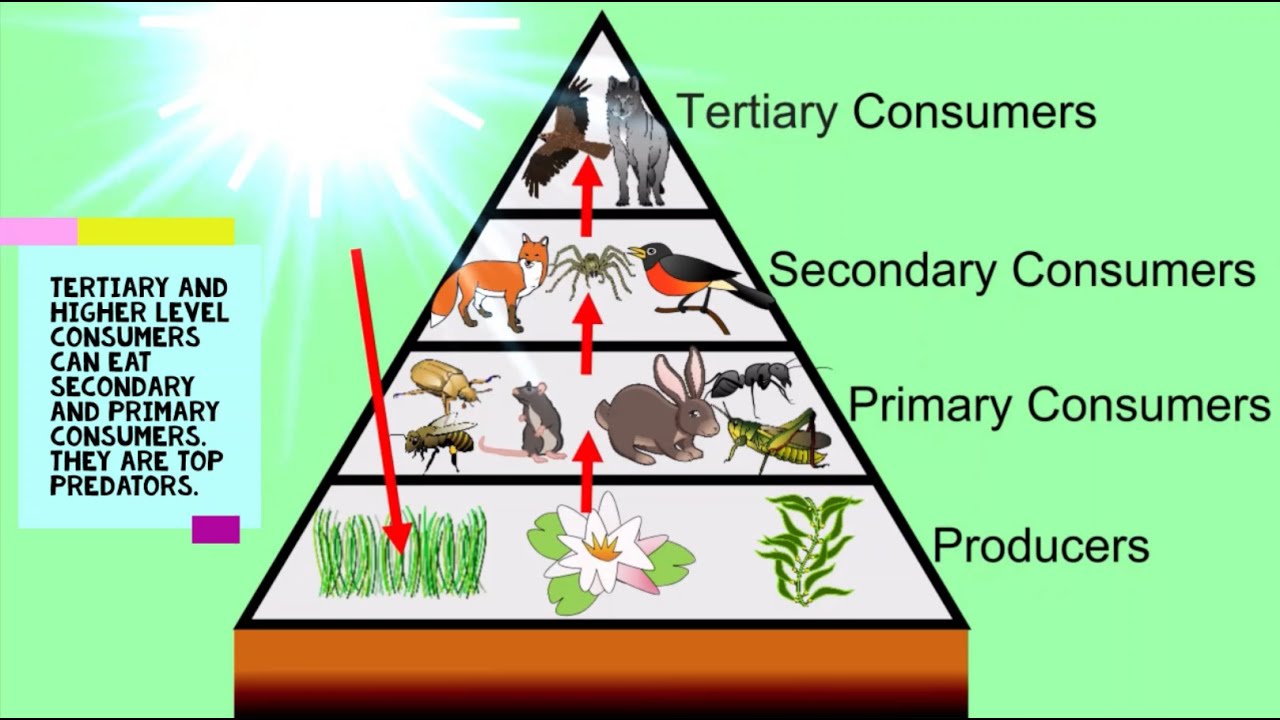
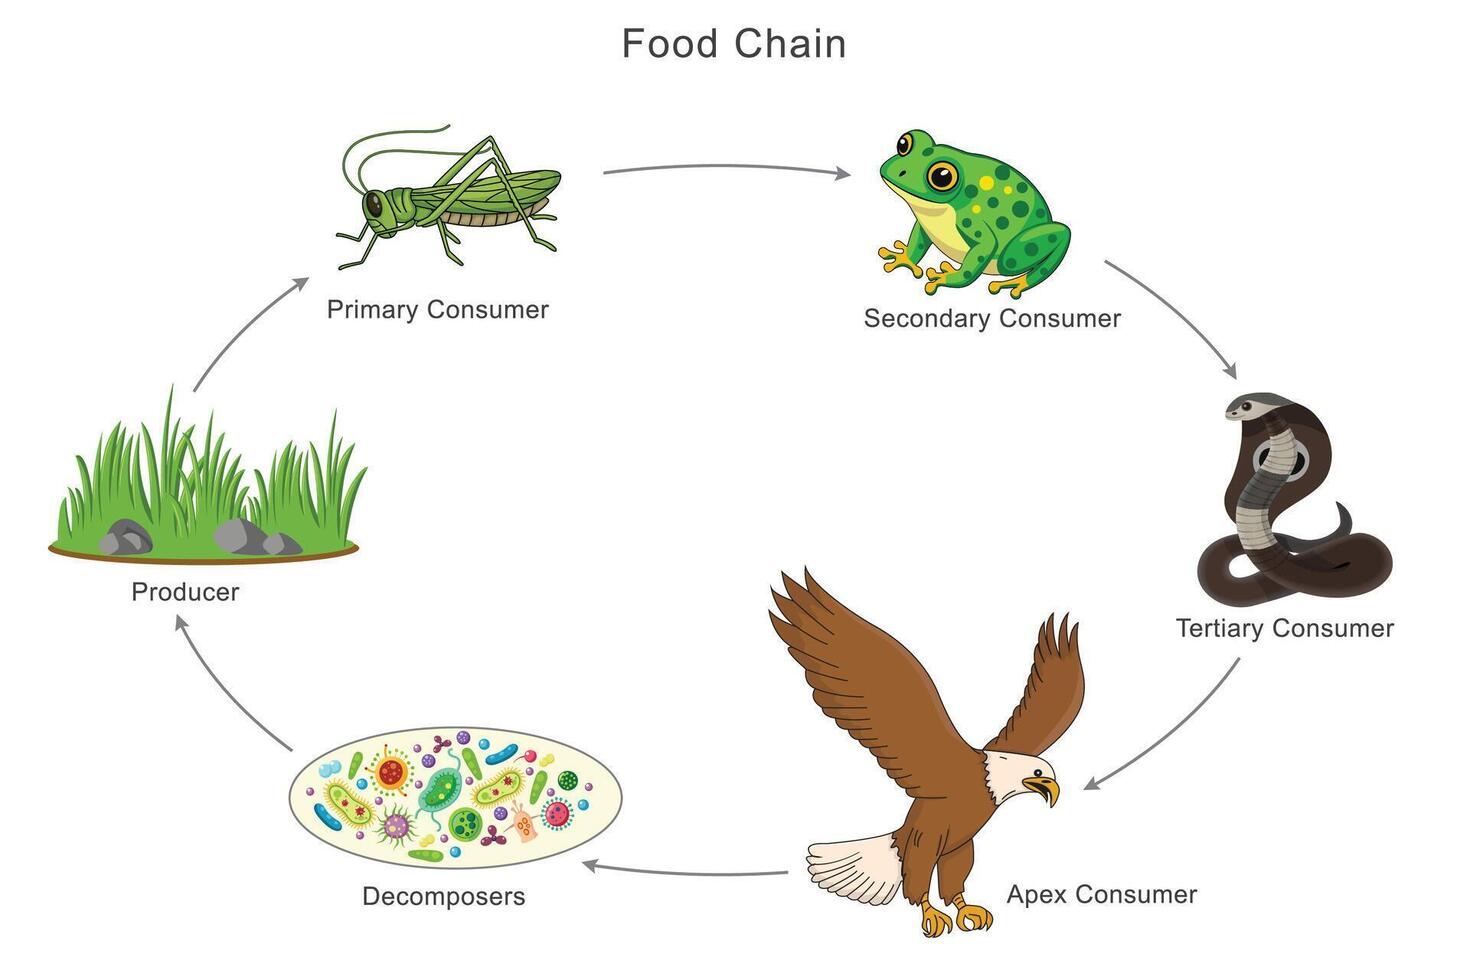
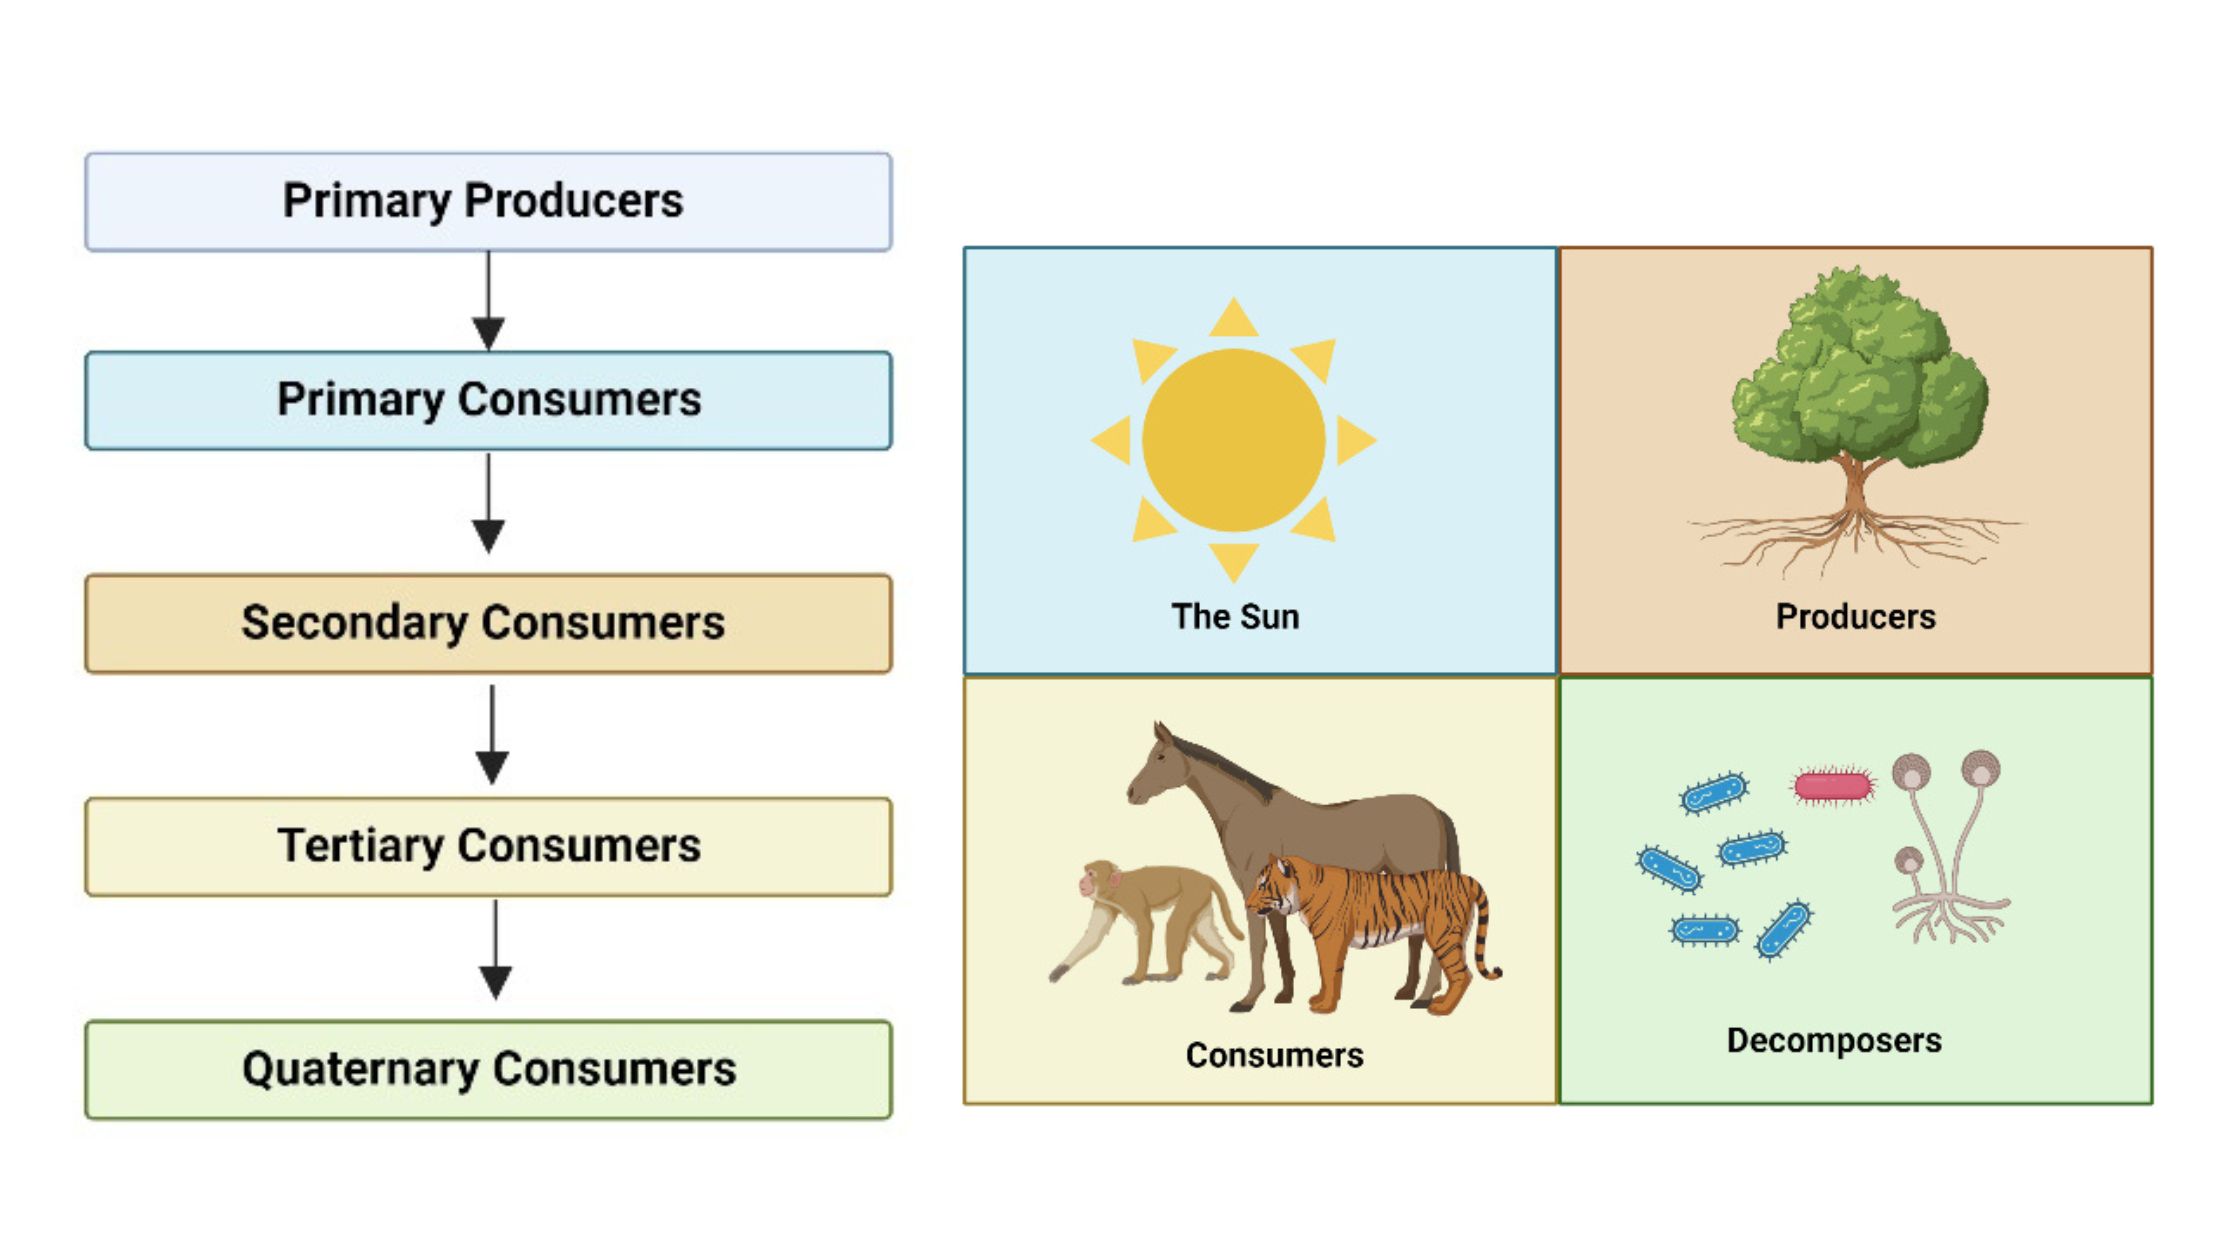
Primary consumers are organisms that feed directly on producers, which means plants, algae, and photosynthetic bacteria. They occupy the second trophic level and serve as the critical energy bridge between autotrophs and the rest of the food web. Without them, energy captured from sunlight by producers would never reach predators, scavengers, or decomposers. The group is far more diverse than most people assume. It includes large grazers like bison and elephants, small insects like grasshoppers and caterpillars, aquatic filter-feeders like zooplankton and mussels, and detritivores like earthworms that consume dead plant material. Each plays a distinct role in nutrient cycling and energy transfer.
Unlocking The Secrets Of Primary Consumers The Unsung Heroes Of The Food Chain
What makes primary consumers ecologically significant goes beyond simply being herbivores. They regulate plant community composition through selective feeding. Deer browsing on understory vegetation, for example, determines which plant species dominate a forest edge. Without that pressure, certain fast-growing species can outcompete slower ones and reduce biodiversity. This is called herbivore-mediated competition, and it is one of the most important dynamics in terrestrial ecosystems. Another thing most people miss is that primary consumers are not just passive eaters. Many have co-evolved specialized digestive systems. Ruminants like cattle have multi-chambered stomachs housing symbiotic bacteria that break down cellulose. Termites rely on protozoan and bacterial partners in their gut to digest wood. These relationships mean the consumer and its microbiome function as a single ecological unit, and disrupting one affects the other. Energy transfer between trophic levels follows a general rule of roughly 10 percent efficiency. That means consuming a kilogram of plant material typically yields about 100 grams of consumer biomass. The rest is lost as metabolic heat, waste, or undigested material. This inefficiency explains why top predator populations are always smaller than herbivore populations, and why ecosystems can support far more grazers than apex carnivores.
When I first started studying grassland herbivore dynamics, I ran into a practical problem that textbooks never really prepare you for. We were tracking elk movement and feeding patterns using GPS collars, but the data showed them spending unusual amounts of time in areas with sparse vegetation. At first we thought the tracking was faulty. It turned out the elk were supplementing their diet with mineral licks hidden in those spots, which meant their forage selection could not be interpreted from location data alone. We had to combine the collar data with direct observation and soil sample analysis to understand what was actually driving their behavior. That project taught me that primary consumer ecology requires multi-method approaches. You cannot rely on a single data source.
Get the Full Details
How to Study Primary Consumer Populations
Field research on primary consumers involves several standard techniques. Direct observation works for large, visible herbivores but becomes impractical for small invertebrates or aquatic species. Camera traps are useful for monitoring grazing patterns but cannot capture diet composition on their own. Pellet counts give you presence data and relative abundance, though they require species-specific conversion factors to estimate actual population numbers. For aquatic systems, net sampling of zooplankton and benthic macroinvertebrates is the standard method, though sampling depth and mesh size significantly affect results. Stable isotope analysis has become a powerful tool in recent years. By measuring carbon and nitrogen isotope ratios in consumer tissue, researchers can trace exactly what plants an herbivore has been eating over weeks or months. This reveals dietary shifts that direct observation would miss, especially for nocturnal or cryptic species. The method is expensive and requires lab access, but it provides data that other techniques simply cannot match. I also learned the hard way that seasonal variation drastically affects every measurement. In temperate zones, primary consumer biomass peaks in late summer but drops sharply after the first frost. If your sampling schedule misses that window, your density estimates can be off by a factor of two or more. Always plan your fieldwork around the specific life cycle of your study species, not your own convenience.
Common Misconceptions
One widespread error is treating all herbivores as ecologically equivalent. A grasshopper and a giraffe both eat plants, but their impact on ecosystem structure is vastly different. Large herbivores are ecosystem engineers. They create gaps in vegetation, disperse seeds through their droppings, and cycle nutrients across wide areas. Small herbivores tend to have more localized effects but can be extraordinarily abundant and reproductively fast. Both matter, but they operate on different scales and require different management approaches. Another misconception involves detritivores. Earthworms, millipedes, and many insect larvae consume dead plant matter rather than living tissue. Some classification systems place them outside the primary consumer category entirely, grouping them with decomposers. Ecologically, however, they function as primary consumers because they occupy the same trophic level and transfer energy from plant biomass to higher levels. The distinction matters mostly for terminology, not for understanding energy flow. The 10 percent rule is also frequently misunderstood as a fixed law. In reality, energy transfer efficiency varies between 5 and 20 percent depending on the ecosystem. Aquatic food chains often show higher efficiency because phytoplankton are more easily digested than terrestrial plant cell walls. Temperate forests tend to fall on the lower end because lignin and cellulose are harder to break down.
Limitations and Where This Framework Falls Short
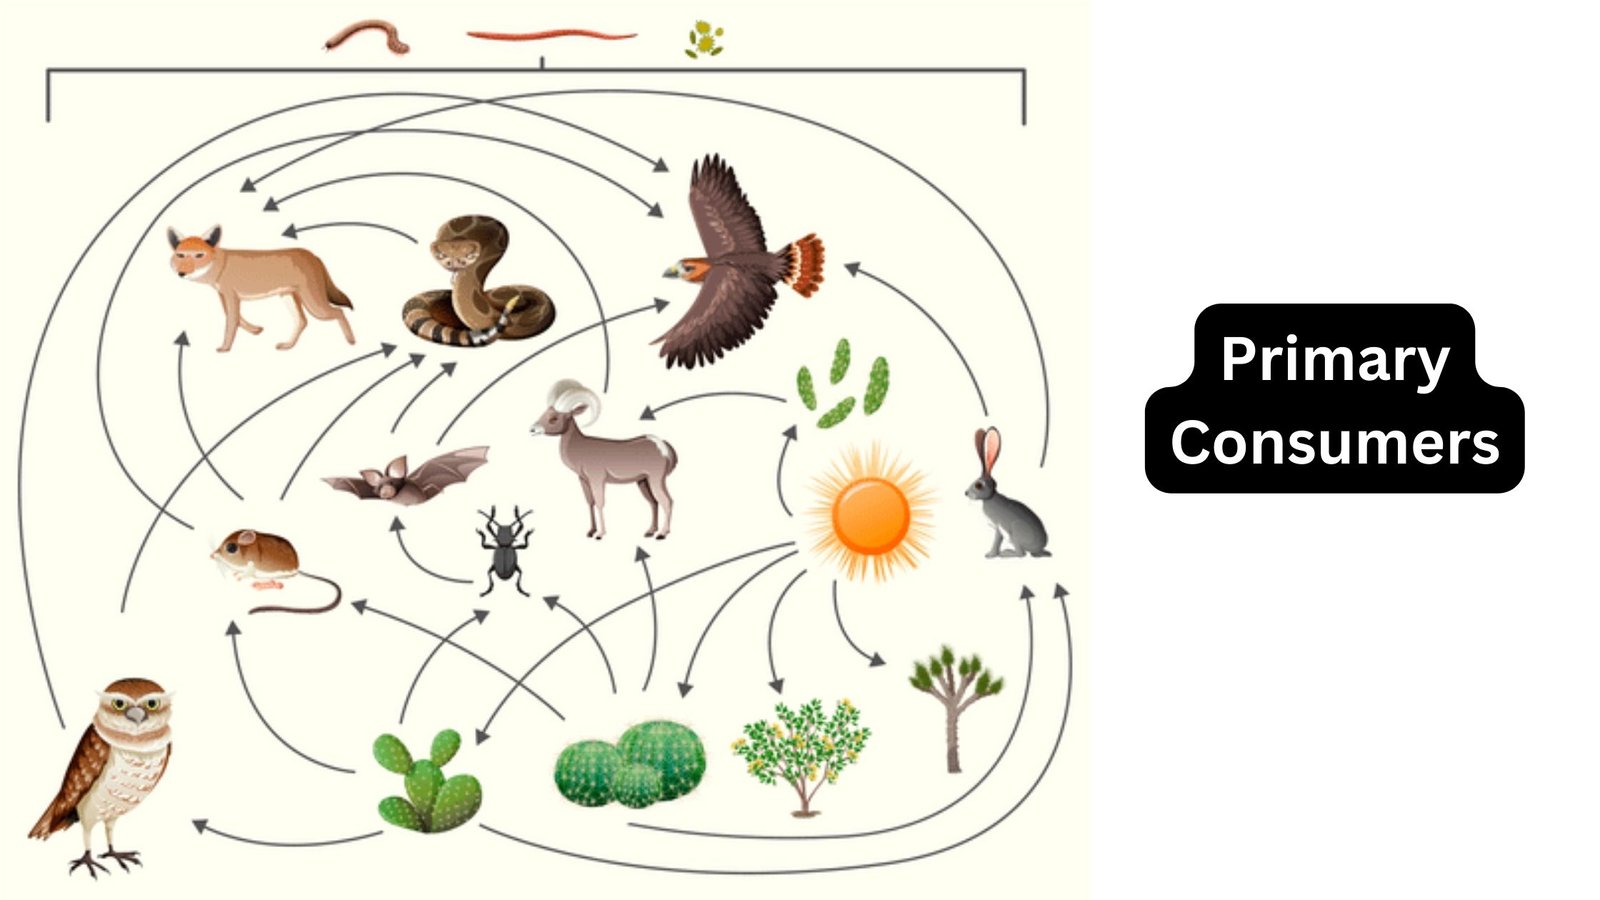
The trophic level model that places primary consumers at the second rung is useful but incomplete. Omnivores complicate the picture entirely. Bears, birds, and many insect species feed on both plants and animals, occupying multiple trophic levels simultaneously. Forced classification into a single level distorts reality. Modern ecology increasingly uses food web networks instead of simple linear chains to capture this complexity. Another limitation is that primary consumer dynamics are often overlooked in conservation planning. Most funding and policy attention goes toward predators or charismatic megafauna. Yet herbivore populations frequently determine whether an ecosystem remains productive or collapses. Overgrazing by introduced species like rabbits in Australia or feral goats on islands has caused irreversible vegetation loss in many cases. Understanding primary consumers is essential for restoration work, not just basic ecology. Finally, climate change is altering primary consumer ranges faster than many species can adapt. Shifts in growing seasons affect plant availability, which cascades directly into herbivore reproduction and survival. Studies in the Arctic show that earlier snowmelt is causing a mismatch between caribou calving and peak plant nutrition. The consumers are arriving at the right time, but the food is already past its peak. This phenological mismatch is a growing problem that the traditional trophic model does not easily address.