Photosynthesis Products: What You Actually Get Out of It
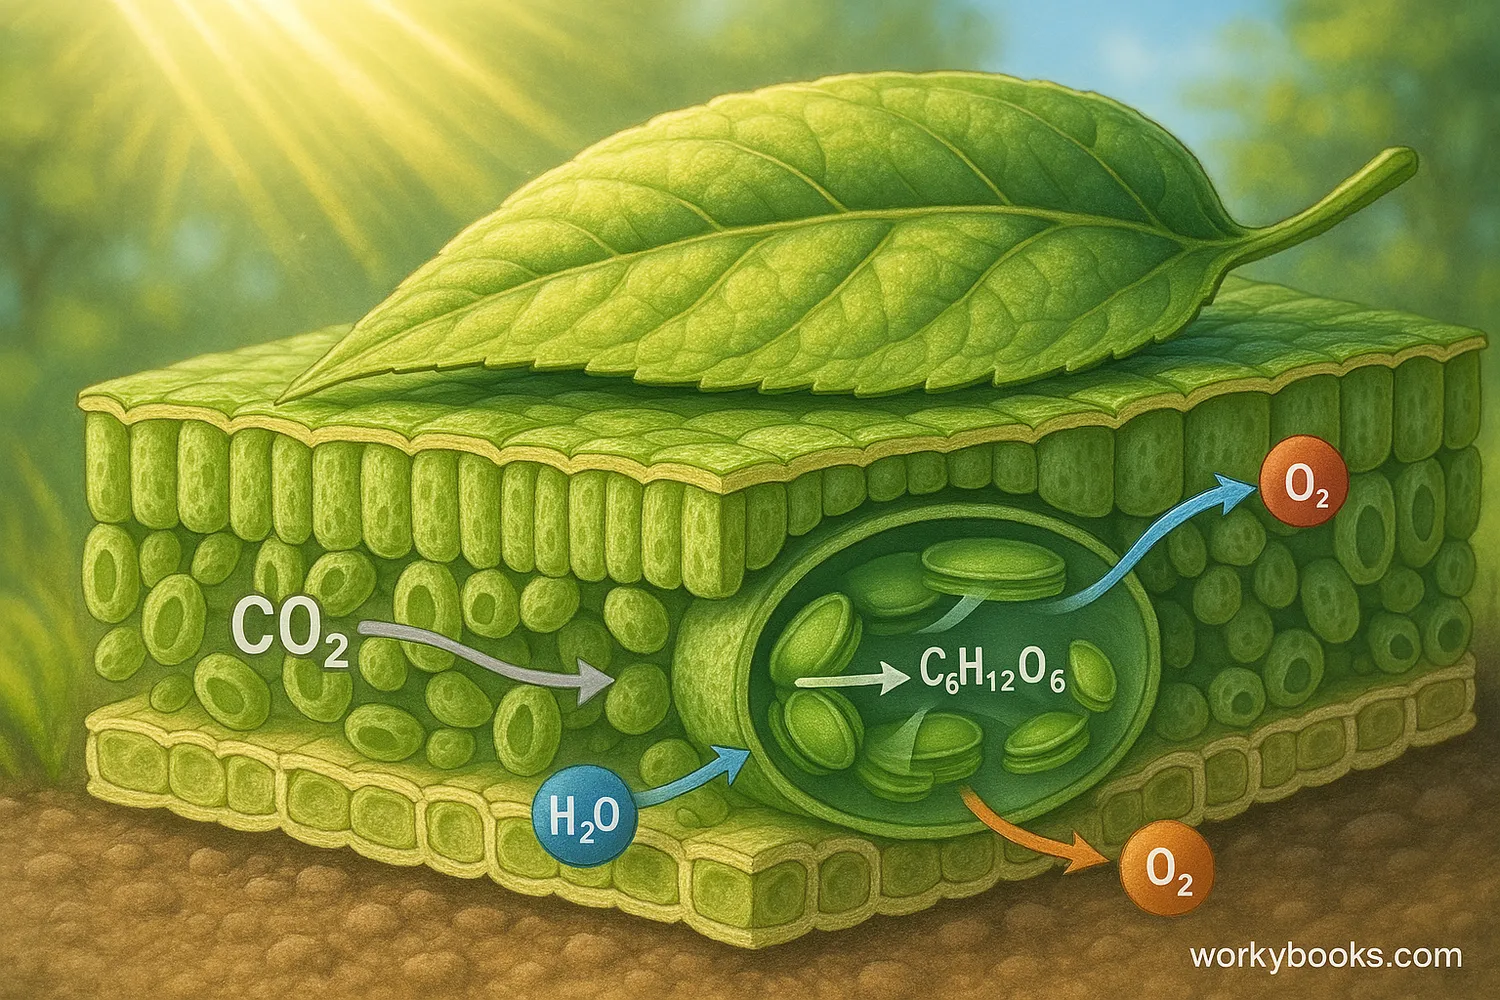
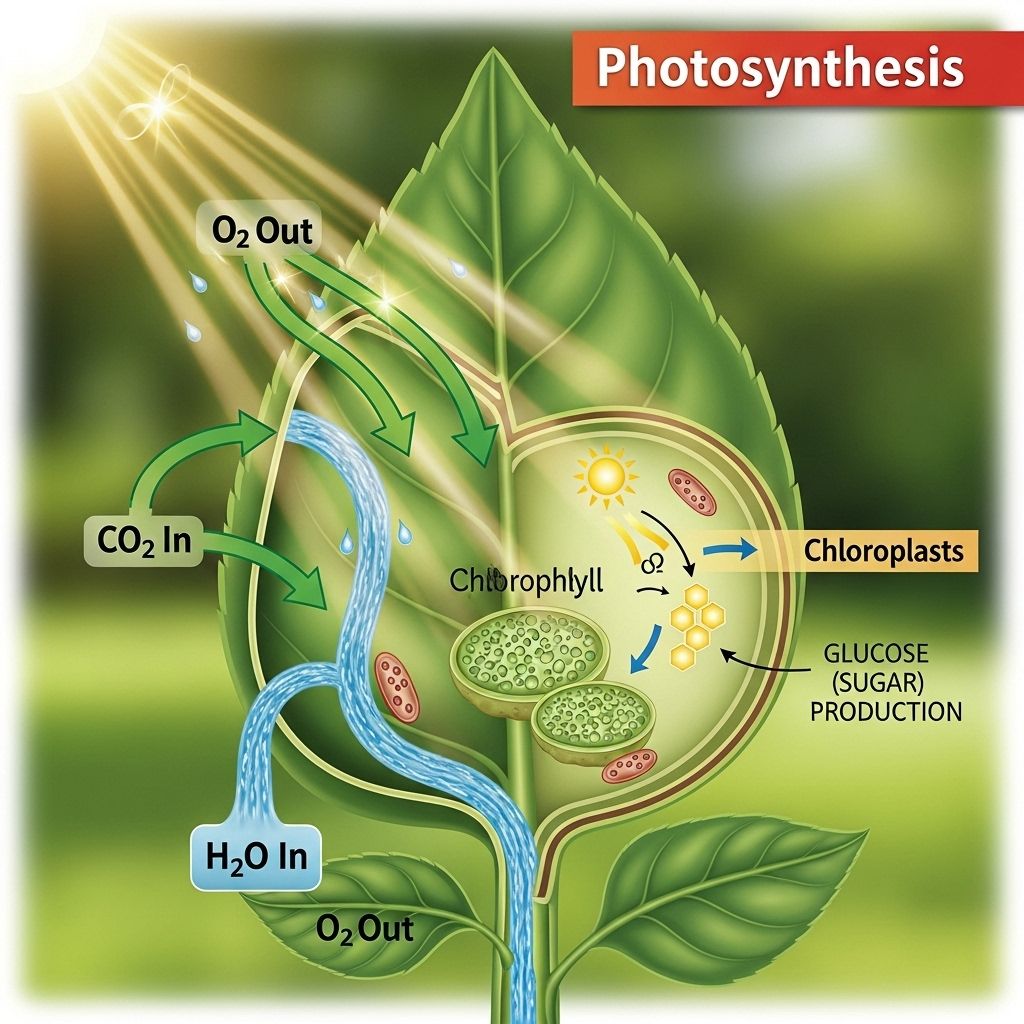
Most people learn the photosynthesis equation in high school biology and forget it by midterms. The short version is that plants take carbon dioxide and water, run them through a light reaction, and spit out glucose plus oxygen. But the actual mechanics are messier than the balanced equation suggests, and there are edge cases that trip up anyone trying to work with real systems instead of textbook diagrams. The primary product is glucose, stored chemically as starch in most plant tissues. Oxygen is a byproduct released through the stomata. The full reaction requires six molecules each of CO2 and water, producing one glucose molecule and six oxygen molecules. Light energy drives the whole process, captured by chlorophyll in the thylakoid membranes of chloroplasts. Here is what the equation actually looks like on paper:
6CO2 + 6H2O + light energy C6H12O6 + 6O2 The glucose does not just sit there waiting to be used. Plants convert it into cellulose for cell walls, starch for storage, or sucrose for transport through the phloem. A single mature oak tree can fix roughly 48 kilograms of carbon dioxide per year, depending on site conditions and age. That translates to about 35 kilograms of glucose produced annually under optimal conditions. I spent two weeks troubleshooting a hydroponic lettuce operation where the growth rate was half of what the literature predicted. The nutrient solution was correct, the pH was stable at 6.2, and the EC read 1.8 millisiemens per centimeter. The plants looked healthy by every visual metric except the actual biomass accumulation. I finally traced the problem to insufficientPAR flux density rather than any nutrient deficiency. The grow lights were rated at 400 micromoles per square meter per second, but the actual measurements at canopy level averaged only 180 due to fixture degradation and mounting height. Once I raised the fixtures and replaced the aging LEDs, growth rates returned to the expected range within ten days.
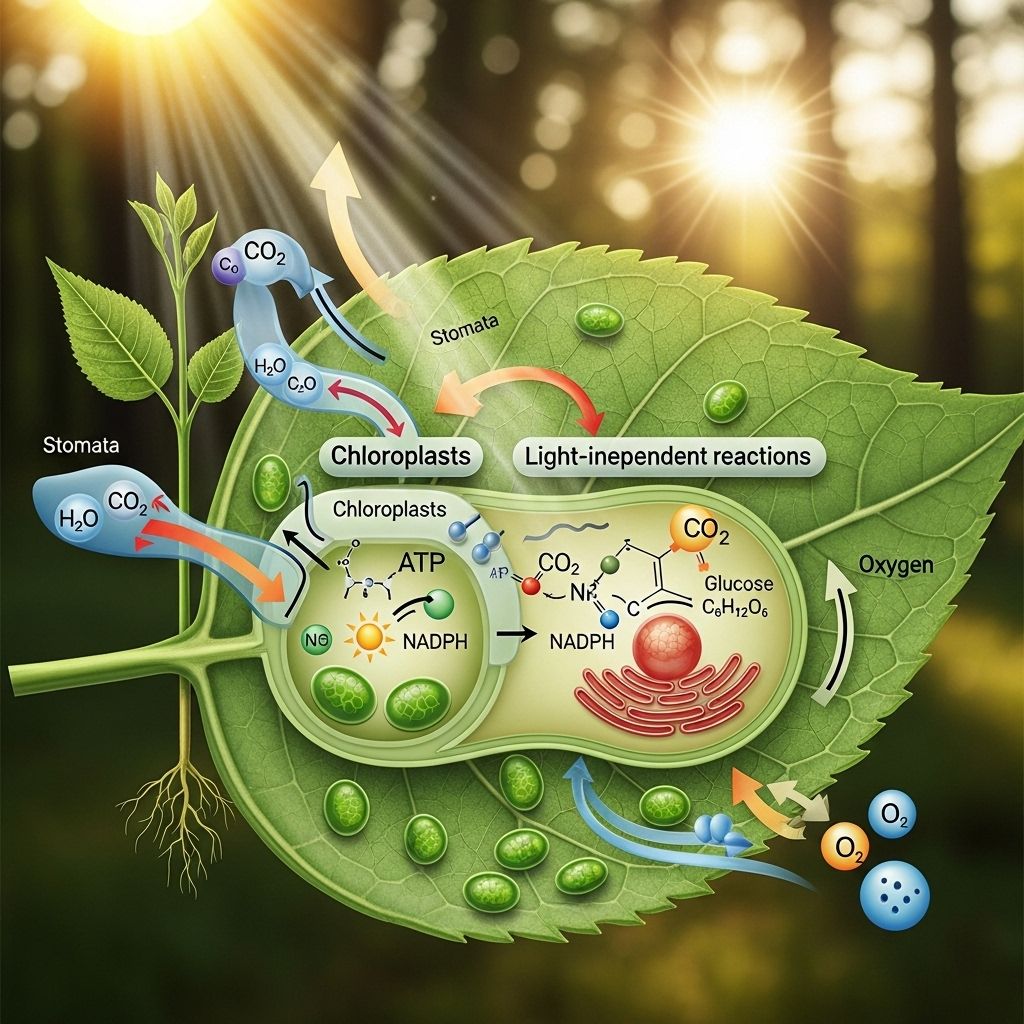
The light-dependent reactions and the Calvin cycle are often taught as separate chapters, but they operate as a tightly coupled system. The thylakoid membrane hosts photosystems II and I, the cytochrome b6f complex, and ATP synthase. Water splitting at photosystem II releases electrons, protons, and oxygen. The electrons travel through the electron transport chain, generating a proton gradient that drivesATP synthesis. NADP+ reductase at photosystem I reduces NADP+ to NADPH using those electrons. The Calvin cycle then uses ATP and NADPH to fixCO2 into glyceraldehyde-3-phosphate, which serves as the precursor for glucose and other carbohydrates. The key enzyme is RuBisCO, which catalyzes the carboxylation of ribulose-1,5-bisphosphate. RuBisCO is notoriously slow, with a turnover number of only about three reactions per second. It also has an affinity for oxygen rather than CO2, leading to photorespiration, which wastes energy and reduces photosynthetic efficiency by up to 25 percent in C3 plants under hot, dry conditions. This photorespiration issue is one of the main reasons C4 and CAM plants evolved alternative carbon fixation pathways. Maize and sugarcane use the Hatch-Slack pathway, concentrating CO2 around RuBisCO using spatial separation between mesophyll and bundle sheath cells. Agave and pineapple use Crassulacean acid metabolism, temporally separating CO2 uptake at night from the Calvin cycle during the day. These adaptations allow photosynthesis to proceed efficiently under conditions that would overwhelm a standard C3 plant.
Get the Full Details
The glucose produced does not immediately become table sugar in the sense we understand it. Plants store it as starch granules in amyloplasts, which can persist for months or years in seeds, tubers, and roots. Sucrose serves as the transport form through the phloem, moving from source leaves to sink organs. A single sugar beet root can accumulate up to 20 percent sucrose by dry weight at harvest, containing roughly 12 kilograms of sugar per plant under typical commercial conditions. One common misconception is that photosynthesis only occurs during daylight hours. The light reactions require photons, yes, but the Calvin cycle can continue for several minutes after light exposure ends, using the remaining ATP and NADPH pools. Some plants, like certain succulents, fix CO2 at night through PEP carboxylase, storing it as malate in vacuoles for use during the day. This temporal separation allows photosynthesis to proceed under conditions where stomatal closure during daylight would limit CO2 intake. The efficiency of photosynthesis is surprisingly low by engineering standards. Only about one to two percent of incident solar energy is converted into chemical energy in glucose. The rest is reflected, transmitted, or lost as heat. Even under optimal laboratory conditions with pure CO2 enrichment, C3 plants rarely exceed three to four percent quantum efficiency. C4 plants can reach five to six percent under the same conditions, but the additional metabolic cost of the CO2 concentration mechanism means the advantage shrinks in cool, shaded environments.
If you are growing plants indoors and want to maximize photosynthetic output, focus on PAR flux density rather than simply increasing light duration. LEDs rated at 600 micromoles per square meter per second are common in commercial operations, but the actual measurements at canopy level often differ by thirty to fifty percent due to fixture degradation, dust accumulation, and mounting height. A simple quantum sensor measuring forty dollars used annually can cut the guessing game short and give you reliable data for adjusting your setup. The oxygen released during photosynthesis does not simply fill the atmosphere uniformly. Most of it is consumed locally by plant respiration, microbial activity in the rhizosphere, and animal respiration in the surrounding ecosystem. Net ecosystem exchange measures the difference between gross photosynthesis and total respiration, and this value determines whether a forest acts as a carbon sink or source. Mature tropical forests can sequester up to 2.5 kilograms of carbon per square meter annually, but this rate declines as the forest ages and approaches equilibrium. Photorespiration becomes a major limitation under rising atmospheric temperatures. As temperature increases, the solubility of CO2 decreases relative to oxygen, and RuBisCO's oxygenase activity increases. This leads to greater photorespiratory losses, reducing photosynthetic efficiency by one to two percent per degree Celsius above the optimal range. Some researchers are engineering RuBisCO variants with higher CO2 affinity, but these efforts have faced challenges with expression levels and stability in heterologous systems.
If you want to observe photosynthesis directly, the classic Elodea bubble counting experiment remains the most accessible method for students. Place a sprig of Elodea in a beaker of water, add a small amount of sodium bicarbonate as a CO2 source, and count the oxygen bubbles released per minute under different light intensities. The bubble rate increases with light intensity until reaching a plateau, at which point another factor becomes limiting. This usually occurs at light saturations around 400 to 600 micromoles per square meter per second for most aquatic plants. The glucose produced serves as the precursor for virtually all organic molecules in the plant. Plants synthesize amino acids from photosynthetic intermediates, fatty acids from acetyl-CoA derived from pyruvate, and nucleotides from ribose-5-phosphate generated in the pentose phosphate pathway. A single leaf can produce up to 30 micrograms of chlorophyll per milligram of fresh weight, capturing roughly 1.5 millimoles of CO2 per square decimeter per hour under optimal conditions. Photosynthesis research continues to evolve with new techniques for measuring gas exchange, chlorophyll fluorescence, and isotope labeling. Infrared gas analyzers measure CO2 uptake and O2 release in real time, with sensitivities down to 0.1 micromoles per mole. Chlorophyll fluorometers measure the efficiency of photosystem II using variable fluorescence, providing insights into photoinhibition and stress responses that gas exchange alone cannot detect.
The byproducts of photosynthesis extend beyond glucose and oxygen. Plants release volatile organic compounds during photosynthesis, including isoprene and monoterpenes, which serve as signaling molecules and protective agents against environmental stress. A single mature tree can emit up to 500 grams of isoprene annually, contributing roughly 12 percent of global biogenic VOC emissions and influencing atmospheric chemistry on a regional scale.