How Cells Actually Store Respiration Energy
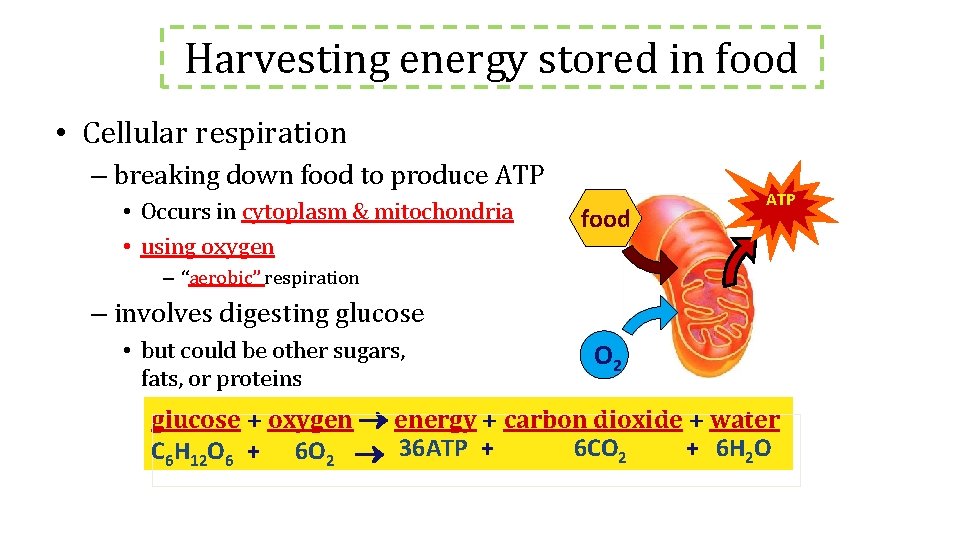
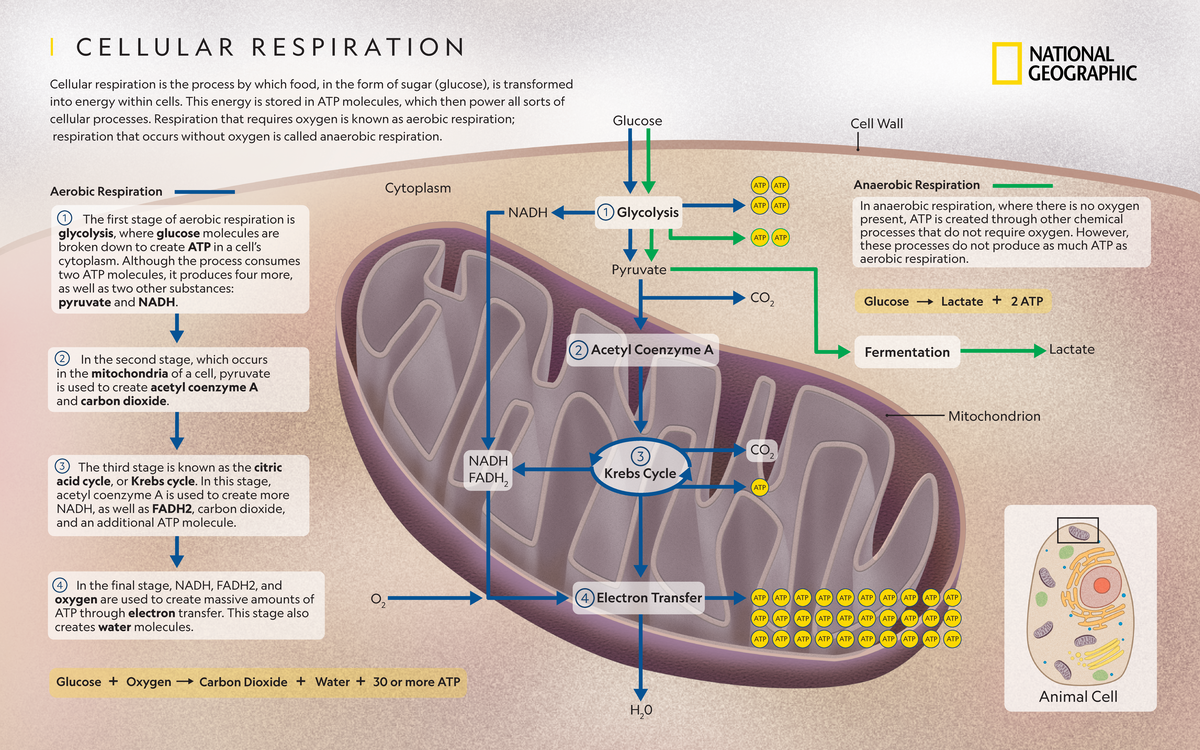
Most people think of cellular respiration as a process that just produces energy and calls it done. It doesn't work that way. The real story is about what happens after the electron transport chain finishes its job. You get protons pumped across the inner mitochondrial membrane, you get a gradient, you get ATP synthase spinning, and then the immediate question becomes where that ATP actually goes and how it's kept around for when the cell needs it later. The short answer is ATP. Adenosine triphosphate. It's the molecule that carries energy in a form the cell can actually use. The three phosphate groups are chained together, and the bond between the second and third phosphate is what stores the energy. When that bond breaks and the terminal phosphate is removed, you get ADP plus a free phosphate, and the released energy powers everything from muscle contraction to active transport across membranes. But here's where it gets more complicated than the textbook version. ATP isn't really a long-term storage molecule. It's more like cash in your wallet. You need it immediately or you lose it. A typical human cell holds maybe two to three millimolar ATP at any given time, and it turns over that entire pool roughly once every minute under normal conditions. That's why cells have backup systems.
In muscle tissue especially, you'll find creatine phosphate hanging around. It's a much faster way to regenerate ATP from ADP. The enzyme creatine kinase shuttles a phosphate from creatine phosphate directly onto ADP, and it happens in milliseconds. That's why you can make a sudden burst of movement before your aerobic respiration even kicks into gear. The problem is creatine phosphate stores last maybe ten to fifteen seconds of max effort before you're running on fumes. After that, it's all about what your mitochondria can sustain. Then there's glycogen. Glucose molecules strung together in branched chains, packed into the cytoplasm of liver and muscle cells. This is the real long-term storage form. Glycogen can hold thousands of glucose units, and when the cell needs more ATP, enzymes break it back down into glucose-1-phosphate, which feeds straight into glycolysis. A single muscle cell can store enough glycogen to keep running for maybe an hour of moderate activity before it runs out. The liver's glycogen is a different story because it's dedicated to keeping blood sugar stable for the rest of the body, not for the liver's own ATP needs. Fat is the heavy lifting. Triglycerides stored in adipose tissue contain vastly more energy per gram than glycogen does. Roughly nine kilocalories per gram compared to about four for carbohydrates. The catch is that mobilizing fat takes time. You need lipases to break triglycerides into free fatty acids and glycerol, the fatty acids have to get transported into the mitochondria via the carnitine shuttle, and then beta-oxidation slowly chops them into acetyl-CoA units that enter the Krebs cycle. This is why sustained, lower-intensity activity is where fat becomes the dominant fuel source. It can't keep up with high-intensity demands because the pathway is just slower.
I ran into a specific problem a few years ago while working with cell culture data. We were measuring oxygen consumption rates in cancer cell lines to figure out their metabolic profiles, and the ATP levels seemed wrong. The cells had normal OCR readings but unexpectedly low intracellular ATP. The issue turned out to be uncoupling protein expression. These cells had upregulated UCP2, which creates a proton leak across the inner mitochondrial membrane. The protons were flowing back through the membrane without going through ATP synthase, so the cell was burning fuel but not actually producing ATP efficiently. It was essentially idling the engine. The workaround was using oligomycin to block ATP synthase and FCCP to fully uncouple, then comparing the reserves to basal respiration. That got us the spare respiratory capacity numbers we actually needed instead of the noise we were seeing before. Another thing that almost nobody explains clearly is the concept of the adenylate energy charge. It's not just about how much ATP you have. It's about the ratio of ATP, ADP, and AMP in the cell. The equation is ATP plus half of ADP, divided by the total adenylate pool. A healthy cell keeps this between 0.8 and 0.95. When it drops below 0.7, energy-dependent processes start failing. The beauty of the system is that AMP acts as a signal. Even a small drop in ATP causes a disproportionately large rise in AMP because of the myokinase reaction that converts two ADP molecules into one ATP and one AMP. That AMP then activates AMPK, which flips on catabolic pathways and flips off anabolic ones. It's an elegant fail-safe that most introductory courses skip entirely. There are also some edge cases worth knowing about. Brown adipose tissue doesn't store energy the same way. It has UCP1, which intentionally uncouples respiration from ATP production to generate heat instead. That's why infants and hibernating animals can maintain body temperature without shivering. The energy from respiration goes directly to thermal output rather than being captured as ATP. If you're studying metabolism in that context, expecting standard ATP yields will give you wildly incorrect numbers.
Get the Full Details
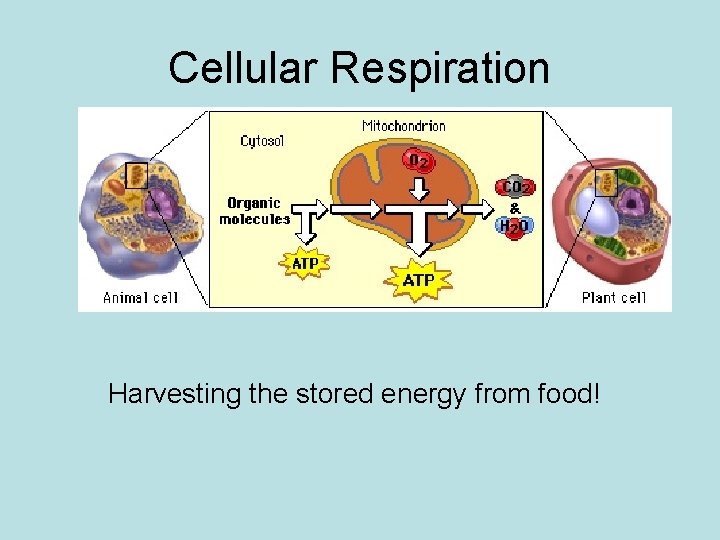
Another practical limitation is that some cells simply can't store much energy at all. Red blood cells lack mitochondria entirely, so they rely on anaerobic glycolysis for ATP. They can't store glycogen either, which means they're running on borrowed time with whatever ATP is currently available. Neurons are similarly constrained because they can't store glycogen in useful amounts and depend almost entirely on continuous glucose delivery from the bloodstream. That's why even a brief interruption of blood flow causes cognitive dysfunction within seconds. The takeaway isn't complicated. Respiration produces ATP, and the cell manages that ATP through a hierarchy of short-term and long-term storage molecules depending on what it needs and how quickly it needs it. Glycogen for hours. Fat for days. Creatine phosphate for seconds. ATP itself for moments. Each layer has its trade-offs in terms of storage density, mobilization speed, and metabolic cost. Understanding which layer is doing the work in any given situation is usually more useful than memorizing the individual reactions.