The Equation Is Simple, But The Biology Isn't
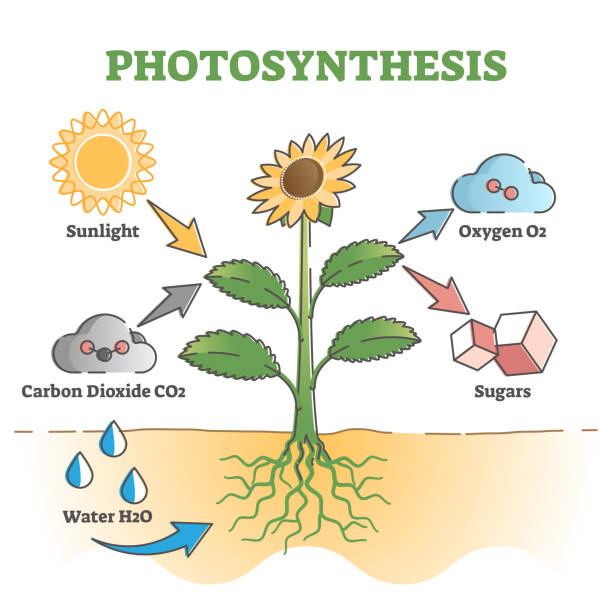
Carbon dioxide plus water, light energy in, glucose and oxygen out. That is the summary formula you see in every textbook. 6CO + 6HO + light CHO + 6O. It is clean on paper. It is also deeply inadequate if you actually try to use it to understand what happens inside a leaf, or if you are working in agriculture or controlled environment growing and need to predict output. Unlocking The Power Of Life Deciphering The Magic Of Photosynthesis Formula requires looking past the balanced equation and into the two phases where the real work happens. The light-dependent reactions and the Calvin cycle are not a single process. They operate on completely different timescales, in different parts of the chloroplast, and respond differently to environmental stress. Treating them as one unit is the most common mistake I see people make.
What Actually Happens In The Chloroplast
Light hits the thylakoid membranes. Photosystem II splits water. Electrons move through the electron transport chain. Protons pile up in the thylakoid lumen. ATP synthase spins and makes ATP. NADP+ gets reduced to NADPH. This all takes milliseconds. The Calvin cycle, which actually fixes carbon, runs on a completely different clock. Rubisco grabs CO and slaps it onto RuBP. The resulting 6-carbon compound immediately splits into two 3-PGA molecules. ATP and NADPH from the light reactions convert those into G3P. Some G3P exits as glucose precursor. Most of it recycles back to regenerate RuBP so the cycle keeps turning. Here is the part most people miss: Rubisco is terrible at its job. It has a slow turnover rate — about 3 carbons fixed per second per active site. Compare that to most enzymatic reactions which process thousands of molecules per second. Rubisco also confuses oxygen for carbon dioxide. When O binds instead of CO, you get photorespiration, which burns energy and releases previously fixed carbon. This is not a edge case. In hot, dry conditions with stomata partially closed, photorespiration can consume up to 50 percent of the fixed carbon in C plants like wheat and rice.
Why The Standard Equation Fails In Practice
I spent several years working with plant physiology data in controlled environment agriculture. The first time I tried to model biomass accumulation using just the standard photosynthesis equation, the numbers were wildly off. Actual yields were 30 to 40 percent lower than predicted. The problem was that the equation assumes ideal conditions — saturating light, optimal temperature, unlimited CO, no water stress. Real leaves never see all of those at once. The workaround I ended up using was incorporating the Farquhar-von Caemmerer-Berry model. It accounts for Rubisco limitation versus RuBP regeneration limitation, temperature dependence of enzyme kinetics, stomatal conductance, and the photorespiratory compensation point. It adds significant complexity but it is the only way to get predictions that match observed growth rates. If you are just studying for a biology exam, the simple formula is fine. If you are designing a grow operation or modeling crop yield under climate stress, you need the mechanistic version. Another practical issue is that the balanced equation implies a 1-to-1 relationship between CO consumed and glucose produced. In reality, the stoichiometry is messy. Producing one molecule of glucose requires 18 ATP and 12 NADPH, not the simplified ratios the basic equation suggests. The light reactions produce ATP and NADPH inroughly a 1.28-to-1 ratio through cyclic and non-cyclic electron flow, and the Calvin cycle demands exactly 1.5 ATP per NADPH. Plants constantly adjust this balance through state transitions and alternative electron sinks like the water-water cycle.
Get the Full Details

C4 And CAM Complicate Everything Further
If you work with corn, sugarcane, or succulents, the standard formula does not apply at all. C4 plants like maize spatially separate the initial CO capture from the Calvin cycle. PEP carboxylase, which has high affinity for CO and zero affinity for O, fixes carbon in mesophyll cells into a 4-carbon compound. That compound shuttles to bundle sheath cells where CO is released at high concentration right next to Rubisco. This suppresses photorespiration almost entirely. The energy cost is higher — C4 plants use extra ATP to run the PEP regenerating pump — but in hot conditions the tradeoff is strongly favorable. CAM plants like cacti and pineapples take temporal separation instead. They open stomata at night to fix CO into malate, store it in vacuoles, then release it internally during the day for the Calvin cycle while keeping stomata closed. This is how they survive in arid environments with extreme water loss constraints. The photosynthesis equation looks the same on paper but the kinetic behavior is completely different from a C3 plant.
Real Limits You Should Know About
Photosynthetic efficiency in real crops peaks around 3 to 6 percent of incident solar energy converted to biomass. The theoretical maximum is sometimes cited at 11 to 12 percent, but that assumes perfect light absorption, no respiratory losses, and optimal CO concentrations — none of which occur outside a laboratory. Under field conditions, even the best crops rarely exceed 2 percent annual efficiency. Light saturation happens at roughly 20 to 30 percent of full sunlight for shade-adapted species and 80 to 100 percent for full-sun plants. Beyond that point, excess light energy causes photoinhibition, damaging PSII and actually reducing carbon fixation until repair mechanisms catch up. The other hard constraint is temperature. Rubisco kinetics follow Q10 relationships, meaning reaction rates double with every 10°C increase — up to a point. Above roughly 35°C for C3 plants, enzyme denaturation and increased photorespiration cause net photosynthesis to decline sharply. C4 plants tolerate higher temperatures because PEP carboxylase is less temperature-sensitive and the CO concentrating mechanism dampens photorespiration. This is why crop zone maps shift the way they do under warming scenarios. If you need a practical approach for estimating photosynthetic output without running a full Farquhar model, starting with light-response curves measured on your specific species under your specific conditions will save you more time than any textbook formula. Measure net CO uptake at varying irradiance levels, find the light compensation point and saturation point, then fit a non-rectangular hyperbola. It takes about an hour with a portable gas exchange system and gives you parameters that actually predict real-world performance.