Chemical Energy In Biological Systems Is Just Electron Transfer With A Payoff
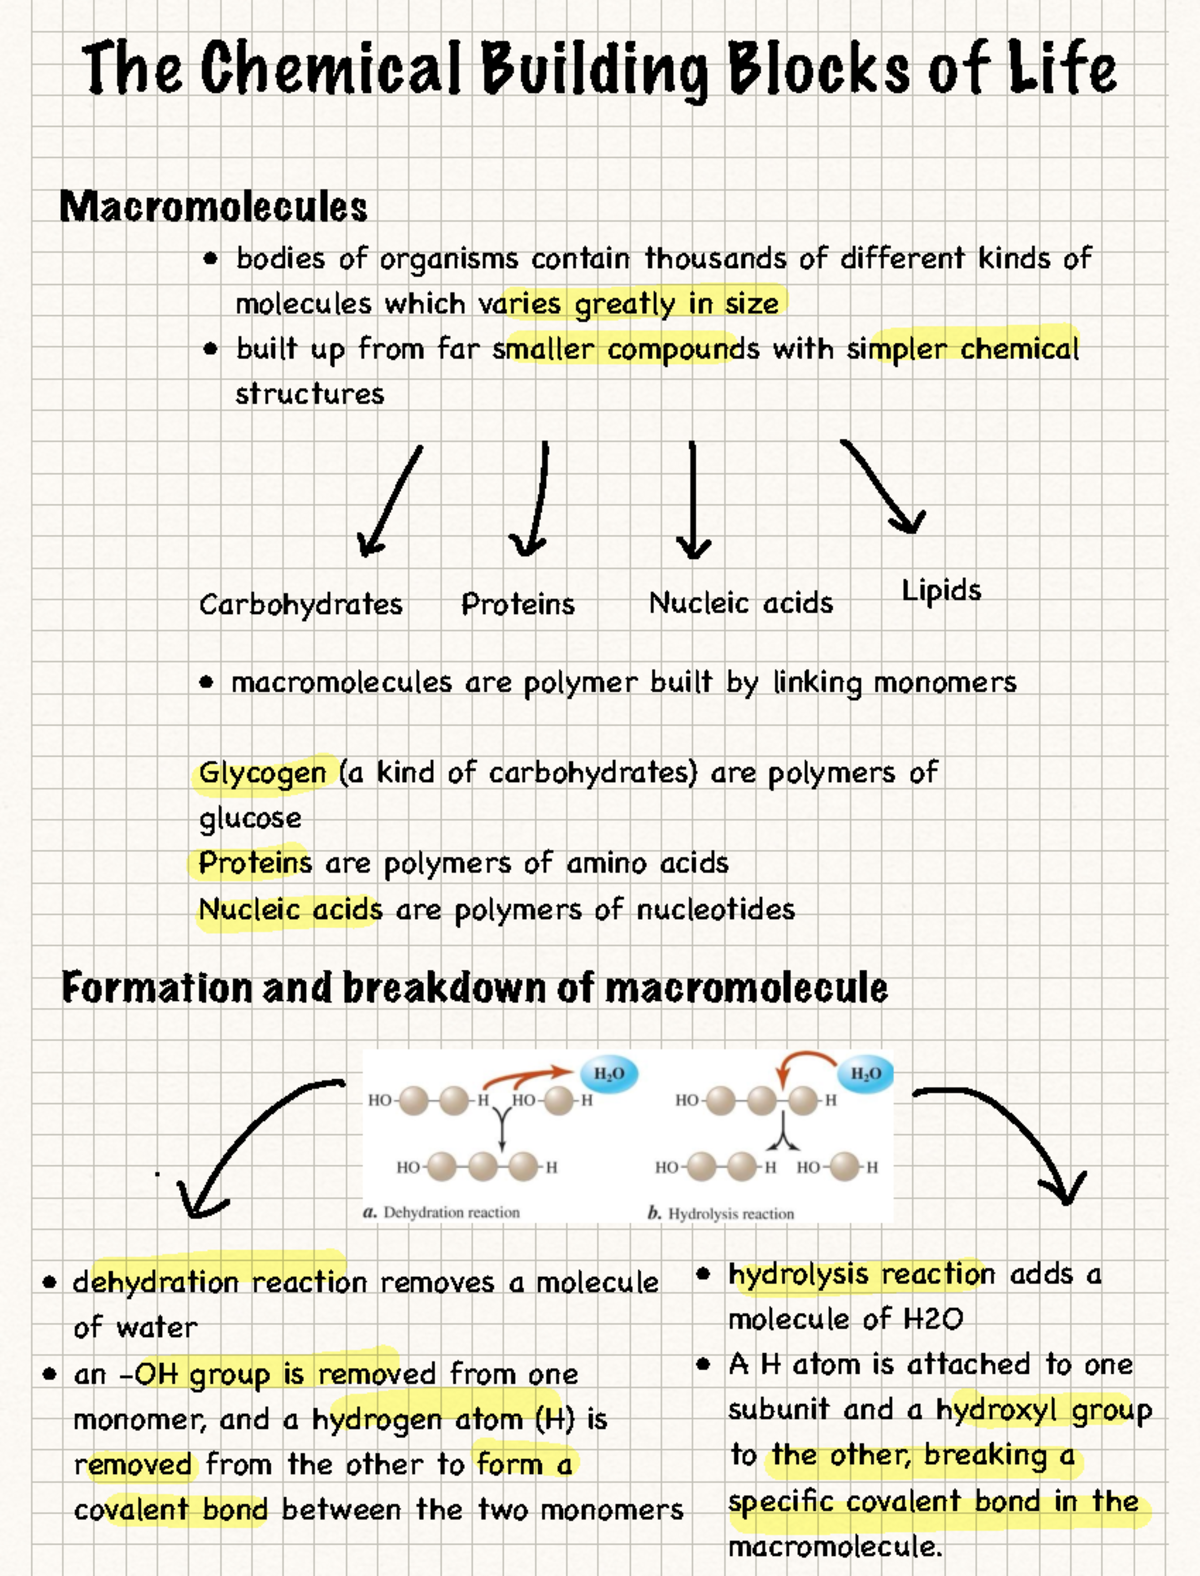
Most people think of "chemical energy" as something abstract you see in textbook diagrams with squiggly arrows and G values. It is not abstract when your cells are trying to stay alive at 3 AM and you have not eaten since noon. Chemical energy in living systems is fundamentally about electrons moving from high-energy states to low-energy states, and whatever is left over gets captured in the form of ATP, NADH, or similar carrier molecules. That is it. Everything else is engineering. If you want to actually understand how this works instead of memorizing the Krebs cycle for an exam, you need to start with the proton gradient. The entire system hinges on maintaining an electrochemical difference across a membrane. The inner mitochondrial membrane is where most of the action happens, and if that membrane is leaky or damaged, everything downstream collapses. I learned this the hard way during a lab course when one of our prepared mitochondrial samples had a compromised membrane due to rough sonication. We kept getting near-zero oxygen consumption rates despite adding ample substrate. The fix was trivial once I realized what was wrong: switch to a glass homogenizer with a loose-fitting Teflon pestle instead of the Dounce homogenizer we had been using, and keep the buffer ice-cold the entire time. Membrane integrity matters more than anything else in prepping functional mitochondria. The building blocks here are not just the classic macromolecules. Yes, carbohydrates, lipids, proteins, and nucleic acids are relevant, but the real building blocks of chemical energy are the cofactors and carrier molecules. NAD+, FAD, coenzyme Q, and ATP itself are the actual currency. The carbon chains in glucose are basically just delivery vehicles for the electrons that end up reducing those carriers. You can survive on a completely fat-based diet with negligible carbohydrate intake because the body simply redirects the electron flow through beta-oxidation into the same proton-pumping machinery. The end result is identical.
Here is something most introductory courses gloss over: the P/O ratio. People memorize that one NADH produces roughly 2.5 ATP and one FADH2 produces roughly 1.5 ATP, but they rarely understand why those numbers are fractional and variable. The truth is that the proton pumping stoichiometry is not clean. Complex I pumps four protons, Complex III pumps four, and Complex IV pumps two. But the ATP synthase requires approximately four protons to produce one ATP, and there is also a proton cost for transporting phosphate and ADP across the inner membrane via the phosphate translocase and adenine nucleotide translocator. Those transport costs eat into the ratio. When I was troubleshooting a respiration assay once, the calculated ATP yield per NADH came out closer to 2.1 instead of the textbook 2.5. The sample had elevated uncoupling protein activity from brown adipose contamination, which dissipated the proton gradient as heat instead of driving ATP synthesis. That is a real phenomenon, not a lab error, but it wrecked the numbers until we identified the contamination. Chemiosmosis is the mechanism, and Peter Mitchell proposed it in the 1960s when the scientific community largely rejected the idea. The concept is simple enough to state in one sentence: a transmembrane proton gradient stores potential energy that ATP synthase converts into the phosphorylation of ADP. The difficulty lies in the details. The proton motive force has two components, the electrical potential difference across the membrane and the pH gradient. In healthy mitochondria, the electrical component is usually dominant, running around 140 to 150 millivolts with the matrix being negative relative to the intermembrane space. The pH difference is typically only about 0.5 to 1 unit, which sounds small but contributes meaningfully to the total driving force. When you look at metabolic pathways, the key insight is that catabolism and anabolism are not separate systems. They are coupled through shared intermediates and carrier molecules. Glycolysis produces NADH and a small amount of ATP. The pyruvate dehydrogenase complex connects glycolysis to the citric acid cycle. The citric acid cycle itself generates most of the NADH and FADH2 that feed the electron transport chain. Oxidative phosphorylation then uses those electrons to regenerate the NAD+ and FAD that the upstream pathways need to continue running. If any part of this chain stalls, the whole thing backs up. NAD+ depletion from a lack of oxygen at the electron transport chain will halt both the Krebs cycle and glycolysis within seconds. That is why anaerobic conditions force cells into fermentation: to regenerate NAD+ without relying on the electron transport chain, even though fermentation yields only 2 ATP per glucose compared to roughly 30 to 32 under aerobic conditions.
The practical side of working with this system involves understanding what can go wrong. Uncouplers are the most common problem in experimental settings. DNP, FCCP, and even certain environmental toxins act as proton ionophores that shuttle protons across the inner mitochondrial membrane, bypassing ATP synthase. The proton gradient dissipates, the electron transport chain runs at maximum velocity consuming oxygen rapidly, but no ATP is produced. The energy is released as heat. This is exactly how thyroid storm and malignant hyperthermia cause dangerous temperature spikes. In the lab, I have seen contaminated buffers with trace amounts of uncoupling agents produce artificially high respiration rates that looked like healthy mitochondria until you measured ATP production and realized nothing was being synthesized. Inhibitors are another category worth knowing about. Rotenone blocks Complex I. Antimycin A blocks Complex III. Cyanide and azide block Complex IV. Each one creates a different bottleneck. With rotenone, NADH accumulates and the Krebs cycle stops, but electrons from FADH2 can still flow through Complex II to ubiquinone and down the chain. With cyanide, everything stops because oxygen cannot accept electrons at the final step. Carbon monoxide acts similarly to cyanide but binds to the heme iron in Complex IV with much higher affinity, which is why CO poisoning is so rapidly fatal even at low concentrations. The hemoglobin binding gets most of the attention, but the direct inhibition of cytochrome c oxidase is equally lethal. For people who want to actually apply this knowledge rather than just pass a test, the useful framework is to think in terms of flux control. The rate of ATP production is not controlled by any single enzyme. It is distributed across multiple steps, with the greatest control often residing in the adenine nucleotide translocator and the phosphate transporter rather than in any single metabolic enzyme. This is called distributed control and it is a concept from metabolic control analysis that most biochemistry courses skip entirely. When I consulted on a project studying exercise metabolism, the initial hypothesis was that phosphofructokinase-1 was the primary rate-limiting step in glycolysis during intense effort. The data showed it was not. The actual control was spread across hexokinase, PFK-1, and pyruvate kinase, with the dominant control shifting depending on oxygen availability and ATP demand. No single enzyme owned the flux.
Get the Full Details
The thermodynamics are also more nuanced than the standard delta G notation suggests. The G of ATP hydrolysis in the cell is nowhere near the standard value of negative 30.5 kilojoules per mole. Inside a living cell, with actual concentrations of ATP, ADP, and inorganic phosphate, the value is typically around negative 50 to negative 60 kilojoules per mole. That difference matters enormously for understanding why certain reactions are reversible in vitro but effectively irreversible in vivo. The citric acid cycle has three irreversible steps, but they are irreversible because of cellular conditions, not because of the intrinsic chemistry alone. If you are studying this for any practical purpose, whether it is nutrition, exercise physiology, or medical research, focus on the regulatory points rather than memorizing every intermediate. The key control points are the pyruvate dehydrogenase complex, isocitrate dehydrogenase, and alpha-ketoglutarate dehydrogenase in the Krebs cycle. At the glycolytic level, PFK-1 is the main regulatory enzyme, sensitive to ATP, citrate, AMP, and fructose-2,6-bisphosphate. The electron transport chain itself is regulated primarily by the availability of ADP, which is called respiratory control. When ADP is abundant, respiration accelerates. When ATP builds up and ADP drops, respiration slows. This is the simplest and most important feedback loop in human bioenergetics. One edge case that causes confusion is the shuttle systems. NADH produced in the cytosol during glycolysis cannot directly cross the inner mitochondrial membrane. The malate-aspartate shuttle and the glycerol-3-phosphate shuttle move the reducing equivalents across, but they do so with different energy costs. The malate-aspartate shuttle transfers electrons to mitochondrial NAD+, preserving the full yield of about 2.5 ATP per cytosolic NADH. The glycerol-3-phosphate shuttle transfers electrons to FAD, yielding only about 1.5 ATP per cytosolic NADH. Muscle and brain predominantly use the malate-aspartate shuttle, while heart and liver rely more on the glycerol-3-phosphate shuttle. This difference affects the total ATP yield from a single glucose molecule and is often overlooked in calculations.
Thermogenin or UCP1 in brown adipose tissue represents a deliberate biological hack on the system. Instead of letting the proton gradient drive ATP synthesis, UCP1 allows protons to flow back into the matrix without passing through ATP synthase. The energy is released as heat. This is not a malfunction. It is an adaptive mechanism for non-shivering thermogenesis, especially important in infants and in adults exposed to cold. The same principle applies to UCP2 and UCP3 in other tissues, though their roles are less clearly defined and may involve regulating reactive oxygen species production rather than heat generation. The bottom line is that chemical energy in human biology is a proton gradient management problem. The electrons come from food, the carriers transport them, the complexes pump protons, and the synthase converts the gradient back into chemical bonds. Every disease of mitochondrial function, every metabolic disorder, and every effect of toxins or drugs ultimately traces back to a disruption at one of these steps. Understanding which step is affected and how the system compensates is more useful than any memorized pathway diagram.