
So You Want To Understand How Meiosis Actually Generates Variation
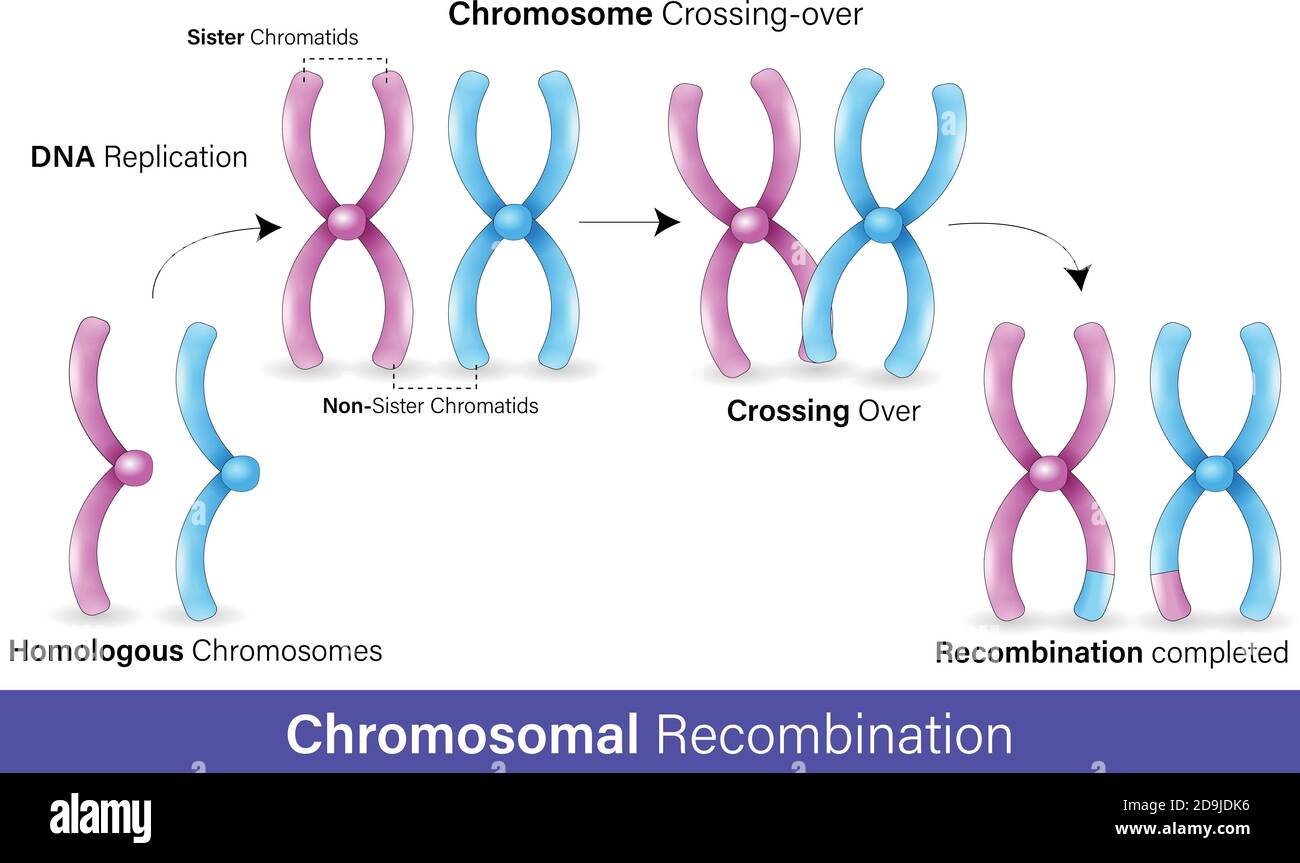
Most textbooks will tell you recombination happens during prophase I and that it creates diversity. They will not tell you how often it actually works correctly in a lab setting, or what happens when your crossover frequency drops to nearly zero and you are staring at a pile of nondisjunction products. I learned that the hard way with a series of Arabidopsis knockouts where the expected recombinant classes simply never showed up. Here is what is actually going on. During the pachytene stage of meiosis I, homologous chromosomes pair up and form the synaptonemal complex. Within that structure, programmed double-strand breaks are introduced by the SPO11 protein complex. Most of these breaks get repaired using the homolog as a template rather than the sister chromatid, which is the whole point. That template-switching event produces either a crossover or a non-crossover product. The crossover is what physically links the homologs together as a chiasma, and without that link, the chromosomes mis-segregate during anaphase I. The genetic diversity part comes from the fact that each crossover shuffles alleles between parental chromosome copies. But here is the thing people routinely miss: the number and position of crossovers is highly regulated. There is a phenomenon called crossover interference where one crossover event reduces the probability of another crossover forming nearby. In most organisms you get roughly one to three crossovers per chromosome arm, never zero and rarely more than five. This regulation is not arbitrary. It exists because too many crossovers destabilizes the bivalent and too few causes nondisjunction.
I spent two solid weeks troubleshooting why my tetrad analysis kept producing mostly parental ditype tetrads with almost no non-parental ditypes. The answer turned out to be that the strain I was working with had a mutation in the MUS81-EME1 resolvase complex, which handles a significant subset of double Holliday junction intermediates. When that pathway is compromised, crossover numbers drop dramatically and the cell falls back on alternative resolution mechanisms that are error-prone. The workaround was straightforward: I backcrossed the strain into a wild-type background and selected for recombinants using a linked visible marker. Within three generations the crossover frequency returned to near-normal levels.
The Mechanism In Practice
Let us get into the actual molecular steps because this is where the real understanding lives. SPO11 creates the double-strand breaks. This is a topoisomerase-like reaction where SPO11 remains covalently attached to the 5' ends of the broken DNA. MRX or MRE11-RAD50-XRS2 complex then resects those 5' ends to produce 3' single-stranded overhangs. Those overhangs invade the homologous chromosome through a process mediated by RAD51 and DMC1, which are meiosis-specific recombinases. DMC1 is particularly important because it biases strand invasion toward the homolog rather than the sister chromatid, something RAD51 alone does not do reliably. Once the invasion happens, you have two possible pathways. The double Holliday junction pathway leads to crossovers. The synthesis-dependent strand annealing pathway typically leads to non-crossovers. In yeast, roughly one-third of repair events become crossovers and two-thirds become non-crossovers. The exact ratio varies by organism and by chromosomal location. Some regions, called hotspots, have much higher recombination rates than others. In humans, the PRDM9 protein determines hotspot location by methylating histone H3 at specific sequence motifs. Without functional PRDM9, as you see in some mouse strains and in a small percentage of human males, recombination hotspots shift and crossover distribution becomes abnormal. This matters because recombination is not evenly distributed across the genome. Centromeric and pericentromeric regions are largely refractory to crossover formation. Telomeric regions can have elevated rates. If you are doing genetic mapping or breeding work, you need to know where your markers sit relative to these hot and cold zones. A marker in a cold zone might appear completely linked to another marker even though they are hundreds of kilobases apart on the physical map.
Get the Full Details

Why This Matters Beyond Textbook Definitions
The critical advantage of recombination is not just that it creates diversity. It is that it creates diversity in a controlled, heritable way while simultaneously ensuring accurate chromosome segregation. These are not separate benefits. They are mechanically coupled. The chiasmata formed by crossovers provide the physical tension that the spindle assembly checkpoint monitors during metaphase I. Without sufficient crossovers, the checkpoint cannot verify proper biorientation and cells either arrest or produce aneuploid gametes. I have seen this play out in real breeding programs where breeders select for tight linkage drag without understanding the underlying recombination landscape. You can end up carrying along large blocks of unwanted genomic material simply because the region between your target gene and the linked marker has very low recombination frequency. In one case, we tracked a disease-resistance locus in wheat and found that the flanking markers were separated by less than 0.5 centimorgans. That means in roughly one out of every two hundred meiotic events you would get a recombinant. Breaking that linkage required screening thousands of progeny over multiple seasons, which is expensive and slow. The faster approach would have been to identify the recombination cold spot first and then choose markers in a more recombinogenic region. Another practical consideration is that recombination rates differ between male and female meiosis in many species. In humans, females have roughly 1.6 times more crossovers than males, and the distribution across chromosomes is also different. Females tend to have more crossovers near telomeres while males show a more central distribution. If you are working with pedigree data or doing linkage analysis, you need to account for this sex-specific difference or your map distances will be systematically wrong.
The Limitations And Where The System Fails
Recombination is not a free lunch. There are real costs and failure modes you need to understand. First, the process is energy-intensive and time-consuming. Meiosis takes significantly longer than mitosis because of the elaborate pairing and recombination machinery. In organisms with large genomes, this can be a genuine constraint on generation time. Second, recombination can be mutagenic. Double-strand breaks, even when repaired correctly, carry the risk of small deletions or insertions at the junction sites. Mis-repair can lead to translocations, especially when breaks occur in repetitive sequences or near structural variants. I once encountered a cell line where a pre-existing inversion led to ectopic recombination between the inverted and non-inverted copies, producing dicentric chromosomes that broke during anaphase. The resulting ring chromosomes caused massive genomic instability that took months to characterize. Third, and this is important for anyone doing practical genetics work: recombination does not occur randomly with respect to selection. Regions of the genome that are under strong selective pressure may show reduced recombination because certain allele combinations are favored and breaking them up would be disadvantageous. This is why supergenes, like the inverted regions controlling mimicry patterns in Heliconius butterflies, remain intact despite being large. The suppression of recombination within the inversion is itself adaptive.
Finally, there is a hard limit on how much diversity recombination can generate in any given population. If the population is small or has gone through a bottleneck, the available allelic variation is limited regardless of how frequently recombination occurs. Recombination shuffles existing variation, it does not create new alleles. For that you need mutation, which operates on a much slower timescale. In practice this means that recombination alone cannot rescue a population that has lost genetic diversity through drift or inbreeding. Conservation biologists deal with this constantly, and the recommendation is always the same: introduce new individuals from other populations to restore variation before recombination has anything meaningful to work with.
What To Actually Do With This Information
If you are doing genetic mapping, start by checking published recombination maps for your organism. Do not assume uniform crossover distribution. Use markers in regions with known moderate to high recombination rates whenever possible. If you are working with a non-model organism without a published map, do a pilot cross with a modest number of progeny and estimate recombination frequencies before committing to a full-scale experiment. If you are studying the molecular mechanism, focus on the resolution of double Holliday junctions. That is where the biggest unanswered questions remain, particularly regarding how cells choose between crossover and non-crossover outcomes at the molecular level. The MUS81, SLX1-SLKX4, and GEN1 nuclease pathways each contribute differently depending on the organism and cell type, and the regulatory signals that direct flux toward one pathway or another are still being worked out. One thing I wish more people understood is that recombination rate itself is a trait that can evolve. There is heritable variation in crossover frequency within populations, and selection can act on that variation. In experimental evolution studies with yeast, populations subjected to stressful conditions often show elevated recombination rates, suggesting that recombination can be upregulated when genetic diversity is most valuable. The mechanism involves stress-response pathways intersecting with the meiotic recombination machinery, though the exact signaling cascades remain incompletely characterized.
The bottom line is that recombination during meiosis is a mechanistically intricate process that serves two essential functions simultaneously: generating genetic diversity and ensuring accurate chromosome segregation. Understanding both functions and their interdependence is what separates someone who can recite the textbook from someone who can actually work with meiotic genetics in a lab or breeding program. The edge cases and failure modes are where the real learning happens.


