What Active Transport Actually Is (Beyond the Textbook)
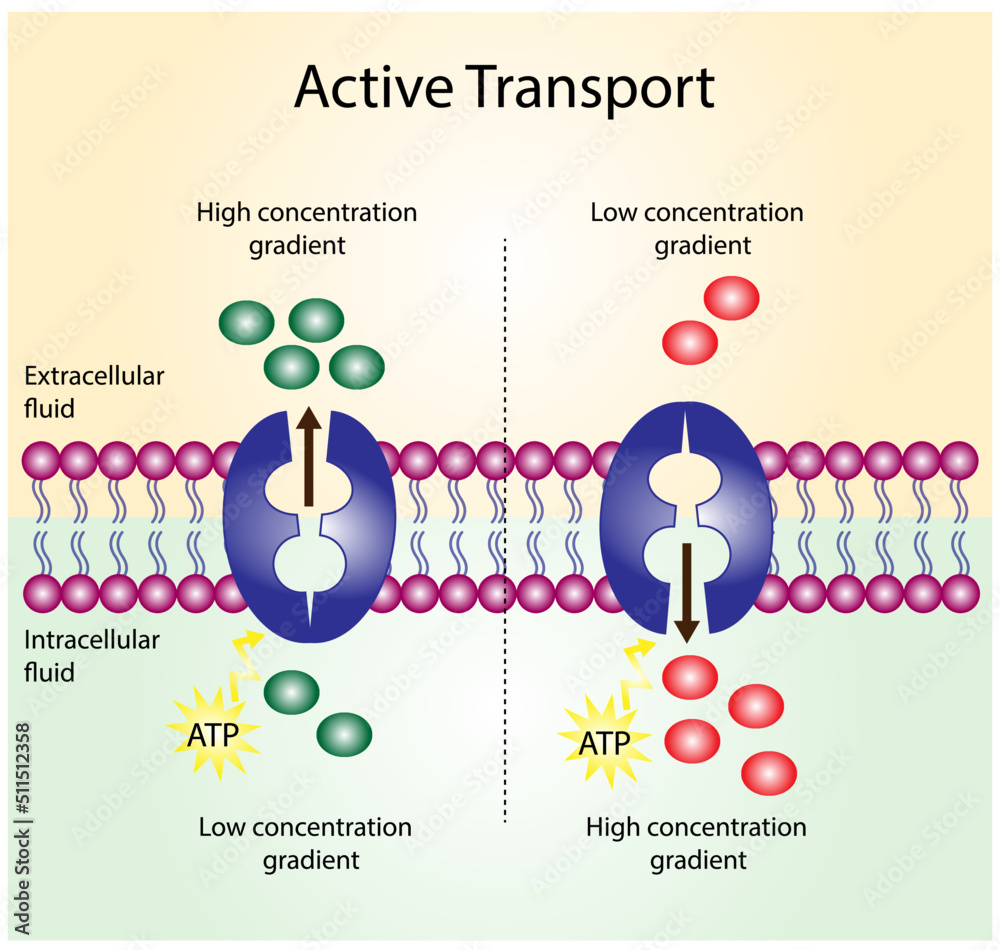
Active transport is the mechanism cells use to move molecules across membranes against their concentration gradient. It requires energy — usually ATP — because without it, those molecules would just diffuse to equilibrium and stay there. The cell doesn't want equilibrium. It wants imbalance. That imbalance is what lets neurons fire, kidneys filter blood, and roots suck nutrients out of soil. I spent a week troubleshooting why a particular cell line stopped accumulating potassium after a routine passage. Turned out the Na+/K+ ATPase was still intact, but the membrane potential had collapsed because we'd been using a media formulation with half the usual magnesium. Magnesium chelates ATP. Without free Mg-ATP, the pump can't hydrolyze it, and everything downstream goes quiet. Weird edge case, took me two days to trace. Just saying — when active transport fails, don't assume the protein is broken. Check the cofactors first.
Unlocking Cellular Secrets Understanding The Essential Process Of Active Transport
There are two main flavors you need to distinguish: primary and secondary. Primary active transport directly hydrolyzes ATP to power the pump. The classic example is the sodium-potassium pump, which shuttles three Na+ ions out and two K+ ions in per cycle. Secondary active transport doesn't touch ATP at all. Instead, it rides the electrochemical gradient established by a primary pump. Think of it as a free ride on someone else's energy bill. The antiport and symport distinction matters more than people give it credit for. In an antiport, the driving ion and the cargo move in opposite directions. In a symport, they go the same way. The sodium-glucose cotransporter (SGLT1) is a symporter you'll see in textbooks a lot. It uses the inward Na+ gradient to drag glucose against its own gradient into intestinal epithelial cells. One molecule of glucose, two sodium ions, same direction. Simple equation, critical physiology.
How the Sodium-Potassium Pump Actually Works
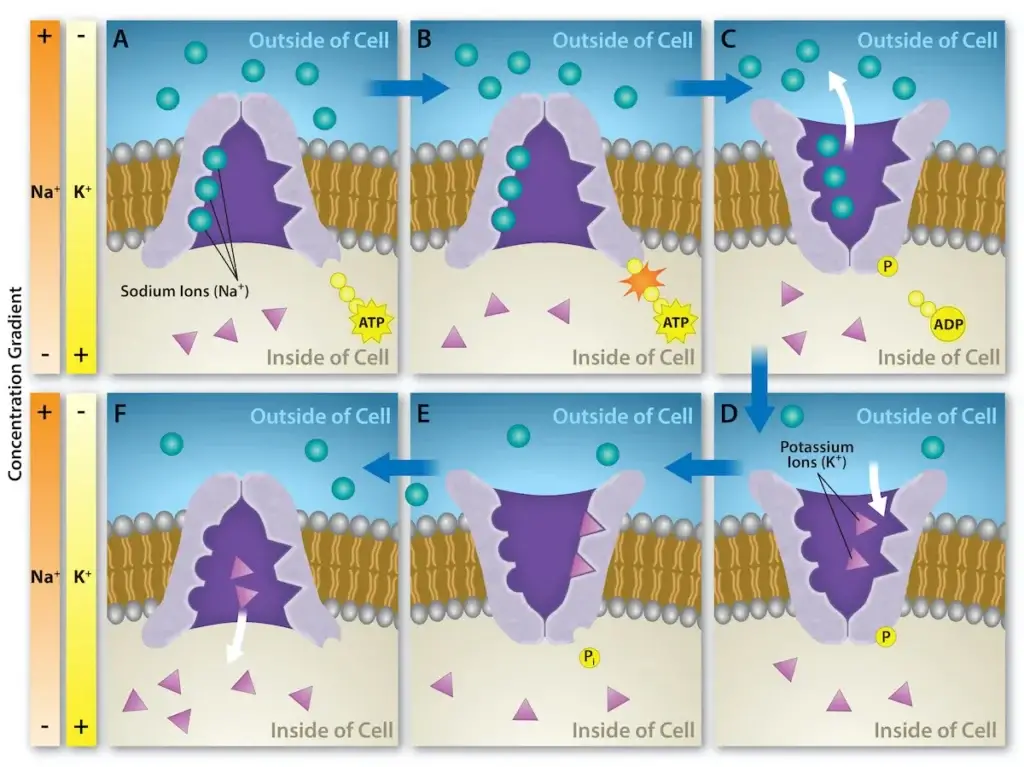
The Na+/K+ ATPase is a P-type pump. "P-type" means it forms a phosphorylated intermediate during its catalytic cycle. Here's the sequence: ATP binds to the intracellular side, the pump phosphorylates itself on a conserved aspartate residue, conformation changes expose the binding sites outward, three Na+ ions released, then dephosphorylation resets the conformation and releases two K+ from the outside back into the cytoplasm. The whole cycle takes about 100 milliseconds under optimal conditions. One thing beginners get wrong is assuming the pump runs at constant speed. It doesn't. The pump's activity is modulated by intracellular Na+ concentration, membrane potential, and hormones like insulin and thyroid hormone. In skeletal muscle during heavy contraction, intracellular Na+ can rise enough to significantly accelerate pump activity. That's not a minor detail — it's how your muscles maintain excitability during a sprint. If the pump couldn't ramp up, you'd cramp out in seconds. I once ran an experiment where we inhibited the pump with ouabain at different extracellular concentrations. The IC50 varied wildly depending on whether the cells were attached to a substrate or in suspension. Adherent cells showed roughly threefold higher sensitivity. The mechanism wasn't clear to me at the time, but I suspect it's related to membrane tension and how ouabain access to its binding site changes with curvature. Worth knowing if you're doing pharmacology work with cardiac glycosides.
Get the Full Details

Secondary Transport and the Proton Gradient Problem
Plant cells and bacteria rely heavily on proton-driven secondary transport. They pump H+ out using ATPase, creating both a pH gradient and an electrical potential across the membrane. Together these form the proton motive force. Nutrients like nitrate, phosphate, and sugars hitch a ride on H+ influx. The catch is that the proton motive force is fragile. A small uncoupler leak — say, from mitochondrial proton slip or a damaged membrane — can dissipate it faster than the primary pump can rebuild it. I've seen cultures lose their ability to take up glucose within minutes of a temperature shock that subtly increased membrane fluidity. The pumps were fine. The gradient just leaked away. If you're working with sensitive cell lines, keep temperature fluctuations under 0.5 degrees Celsius during transport assays. It sounds extreme but it matters.
Common Mistakes When Studying This
Students often confuse facilitated diffusion with secondary active transport because both use carrier proteins and both move molecules against a gradient. The difference is energy source. Facilitated diffusion uses the molecule's own concentration gradient — no external energy input. Secondary active transport couples to an ion gradient that was itself built by primary active transport. Indirect energy use, but energy use nonetheless. Another trap: assuming all active transport is saturable in the same way. It isn't. The Km of the Na+/K+ pump for intracellular Na+ is around 10 millimolar, which means it's half-saturated at normal resting concentrations. But the Km for extracellular K+ is closer to 1-2 millimolar, so under physiological conditions that site is nearly always occupied. If you're modeling this quantitatively, don't treat all binding sites as equivalent. They're not.
When Active Transport Fails Completely
Ischemia is the textbook failure mode. No oxygen, no oxidative phosphorylation, no ATP. The Na+/K+ pump stops within seconds. Intracellular Na+ rises, water follows osmotically, the cell swells. Membrane depolarization triggers glutamate release in neurons, which excites neighboring cells until everything fires synchronously — a seizure at the cellular level. Then the channels run down, calcium floods in, proteases activate, and the cell dies. Reversal is possible if you intervene fast enough. In isolated heart preparations, perfusing with high-potassium solutions can partially restore membrane potential even without full ATP recovery. The trick is that you're giving the pump its substrate (K+) before it has the energy to use it, so the moment ATP returns, the pump can immediately resume work. It's a narrow window — maybe five to ten minutes in mammalian tissue at 37 degrees. Below that temperature the window stretches, which is why organ preservation for transplant uses cold perfusion solutions.
Practical Takeaway
Active transport isn't a single mechanism. It's a family of energy-coupled moves that share one principle: the cell pays to maintain what diffusion would otherwise erase. Whether you're looking at a neuronal sodium channel, a renal glucose transporter, or a bacterial nutrient importer, the question to ask first is always the same — what gradient is powering this, and what's powering that gradient. Follow the energy. It'll tell you where the system is vulnerable.