Why I stopped dreading Punnett squares in biology class
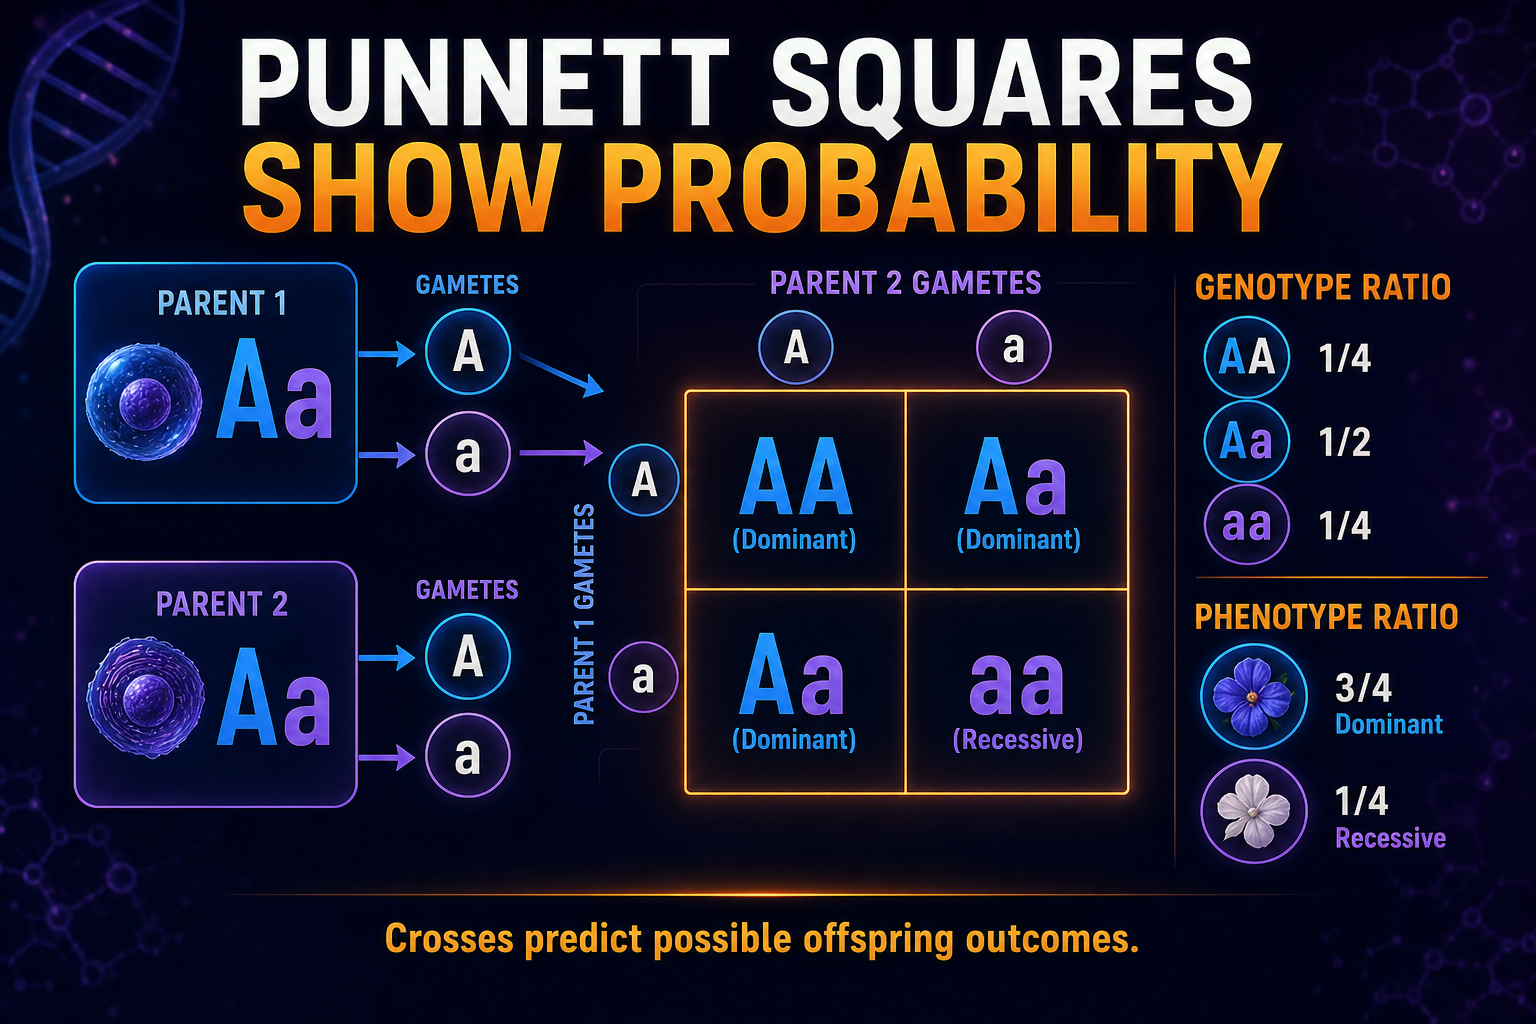
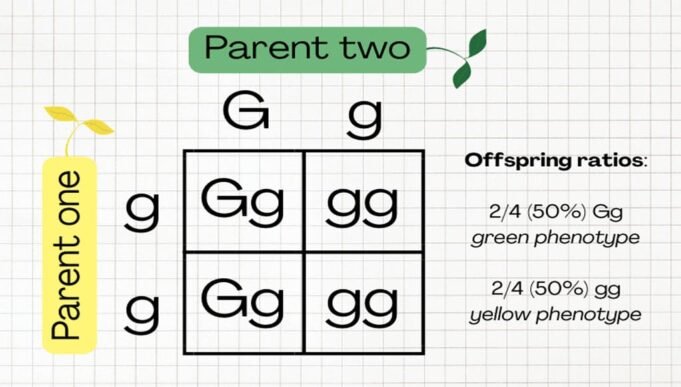
Punnett squares are a visual tool for predicting the probability of offspring genotypes based on parental alleles. That is the textbook definition. In practice they are just a grid where you track allele combinations across two sets of parents. I learned to use them in high school biology during a unit on Mendelian inheritance, and I used them repeatedly while working as a research assistant in a genetics lab during undergrad. The grid is simple. You write one parent's possible gametes across the top. You write the other parent's possible gametes down the left side. Then you fill in each box with the combination from the matching row and column. Each box represents one possible genotype outcome for the offspring.
Unlock The Magic Of Ye Old Unicorn Genetics A Cracking Guide To Punnett Squares
I know the unicorn framing sounds like something a middle school teacher would put on a worksheet, but it is actually a useful way to teach the mechanics without getting bogged down in real organismal complexity before students understand the basic pattern. Here is how I would walk someone through it using a straightforward single-gene example. Let us say you are tracking coat color in a hypothetical unicorn population where the dominant allele H produces a spotted coat and the recessive allele h produces a solid coat. One parent is heterozygous with genotype Hh. The other parent is also Hh. You place H and h along the top. You place H and h down the left side. The four boxes give you HH, Hh, Hh, and hh. That means 25 percent of the offspring are expected to be HH, 50 percent Hh, and 25 percent hh. The spotted phenotype appears in 75 percent of the expected offspring because both HH and Hh carry at least one dominant H allele. The solid phenotype appears in the remaining 25 percent from the hh combination. This works cleanly for any single gene with complete dominance. It also works for codominance and incomplete dominance if you adjust your phenotype interpretation accordingly. It stops being straightforward once you introduce more than two alleles at a single locus or multiple interacting genes.
Where Punnett squares actually fall apart
The most common mistake I see people make is assuming a Punnett square gives you a guarantee for any individual offspring. It does not. It gives you probabilities. If you cross two Hh parents and expect four foals, you might get four hh offspring purely by chance. The square tells you the odds, not the outcome. This is one of those things that is never emphasized enough in introductory courses. A second mistake involves polygenic traits. Height, skin tone, and many behavioral tendencies in organisms are influenced by multiple genes and environmental factors. A Punnett square cannot model that. If someone tries to use one for a trait controlled by five or six genes, the grid becomes unwieldy and the results are misleading. The tool has a narrow zone of reliability, and that zone is basically single-gene Mendelian inheritance with two alleles. I ran into a specific problem once while tutoring a student who was working on a dihybrid cross involving linked genes. They drew a standard 4x4 Punnett square and calculated expected ratios as if the two genes assorted independently. The actual breeding data did not match. The genes were on the same chromosome and close together, so recombination frequency was far below the 50 percent you assume with independent assortment. The workaround was to calculate the recombination fraction from observed data and adjust the expected class frequencies accordingly. In that case, a Punnett square was still useful for organizing the gamete types, but the probabilities had to come from linkage mapping, not from equal quadrant assumptions.
Get the Full Details

Building a dihybrid cross correctly
A dihybrid cross tracks two genes simultaneously. You still use a 4x4 grid, but each parent must produce four types of gametes instead of two. If one parent is AaBb and the other is also AaBb, the possible gametes are AB, Ab, aB, and ab. Place those along the top and down the side. Fill in the boxes. You should get the classic 9:3:3:1 phenotypic ratio if the genes assort independently and show complete dominance at both loci. The trick is making sure you list the gametes correctly before you draw the grid. If you miss a combination or duplicate one, the whole square is wrong. I always recommend writing out the gametes separately first and verifying that the number of unique combinations matches 2^n where n is the number of heterozygous gene pairs. For AaBb that is 2^2 equals 4 gamete types. For AaBbCc it would be 2^3 equals 8, which means an 8x8 grid with 64 boxes. That is when people usually switch to probability multiplication instead of drawing a grid.
Probability multiplication as the faster alternative
For anything beyond a monohybrid cross, multiplying probabilities is faster and less error-prone than filling in a giant grid. You treat each gene independently. The chance of getting aa from an Aa x Aa cross is 1/4. The chance of getting bb from a Bb x Bb cross is 1/4. The chance of getting aabb from both is 1/4 times 1/4, which is 1/16. This approach scales linearly with the number of genes instead of exponentially like the grid method does. I still use Punnett squares when I need to show someone the underlying logic visually. They are better teaching tools for the mechanics of allele segregation. But for actual calculations with three or more genes, I switch to the multiplication rule immediately. It cuts the work down from having to manually fill in 64 or 256 boxes to just a few lines of probability math.
Sex-linked inheritance and the sex chromosome adjustment
Punnett squares handle sex-linked traits without major modification, but you have to remember that males and females produce different gametes when the gene is on the X chromosome. A cross between a carrier female X^H X^h and a normal male X^H Y produces four expected genotype combinations, but the phenotypic ratios differ between male and female offspring. Males inherit only one X allele, so they express whatever allele is on that single X. Females inherit two. This is why X-linked recessive disorders appear more frequently in males. The square itself does not change format, but the interpretation requires you to separate results by sex. I encountered a case where a student drew the grid correctly but reported the overall ratio without separating by sex, which obscured the actual risk for male versus female offspring. The fix was simply to label each box with the sex chromosome contribution and read the results row by row rather than trying to collapse everything into one number.

Testing if observed ratios match expected ratios
Once you have data from an actual breeding or inheritance study, you need to check whether the observed results fit the Punnett square prediction. The chi-square goodness-of-fit test handles this. You take the observed count in each category, subtract the expected count, square the difference, divide by the expected count, and sum across all categories. The resulting value is compared to a chi-square distribution with degrees of freedom equal to the number of categories minus one. If the p-value is above 0.05, the deviation is usually considered consistent with random sampling variation. If it is below 0.05, something may be wrong with your model, such as linkage, incomplete penetrance, or misidentified parental genotypes. This step is often skipped in high school classes because it introduces statistics, but it is the part that actually validates whether your Punnett square analysis is correct. I include it whenever I do real genetics work because a ratio that looks roughly right can still be statistically incompatible with your hypothesis.
When to skip the Punnett square entirely
If the trait involves incomplete dominance, codominance, multiple alleles like the ABO blood group system, or epistasis where one gene masks another, the Punnett square still works for genotypes. You just have to interpret the phenotypes differently. ABO blood types require a 4x4 grid if both parents are type AB, producing nine possible genotype combinations. Epistasis does not change the grid structure, but it changes how you translate genotype to phenotype. The 9:3:3:1 ratio can become 9:3:4 or 12:3:1 depending on the interaction pattern. The square does not break. Your interpretation just has to account for the biological mechanism you are tracking.
Summary of the practical workflow
Identify the parental genotypes first. List all possible gametes for each parent using the 2^n rule. Draw the grid only if the number of gamete types is small enough to make it manageable. Fill in the boxes. Translate genotypes to phenotypes using the correct dominance relationship. Check the ratio against observed data with chi-square if you have real numbers. If the grid gets too large, switch to probability multiplication. The unicorn framing in the original guide title is playful, but the underlying mechanics are the same for pea plants, fruit flies, humans, or whatever organism you are studying. The tool is simple, the limitations are narrow and well-defined, and it remains the standard starting point for any genetics problem before you move into linkage analysis, quantitative trait mapping, or population genetics. I use it when I need clarity. I skip it when I need speed. Both decisions are routine.