How Enzymes Actually Work in the Lab
Enzymes are biological catalysts that speed up chemical reactions by lowering activation energy without being consumed in the process. Most people learn this definition in high school biology and then forget about it for decades. The reality of working with them is more complicated than any textbook chapter suggests. When I first started running PCR assays, I spent weeks frustrated by inconsistent amplification results. The same primer set, same template, same thermocycler settings produced smears one day and clean bands the next. It turned out the Taq polymerase was dying from repeated freeze-thaw cycles, not anything about the reaction chemistry itself. Now I aliquot every enzyme into single-use volumes and store them at minus eighty degrees. The protocol takes an extra ten minutes but eliminates an entire category of variable failure.
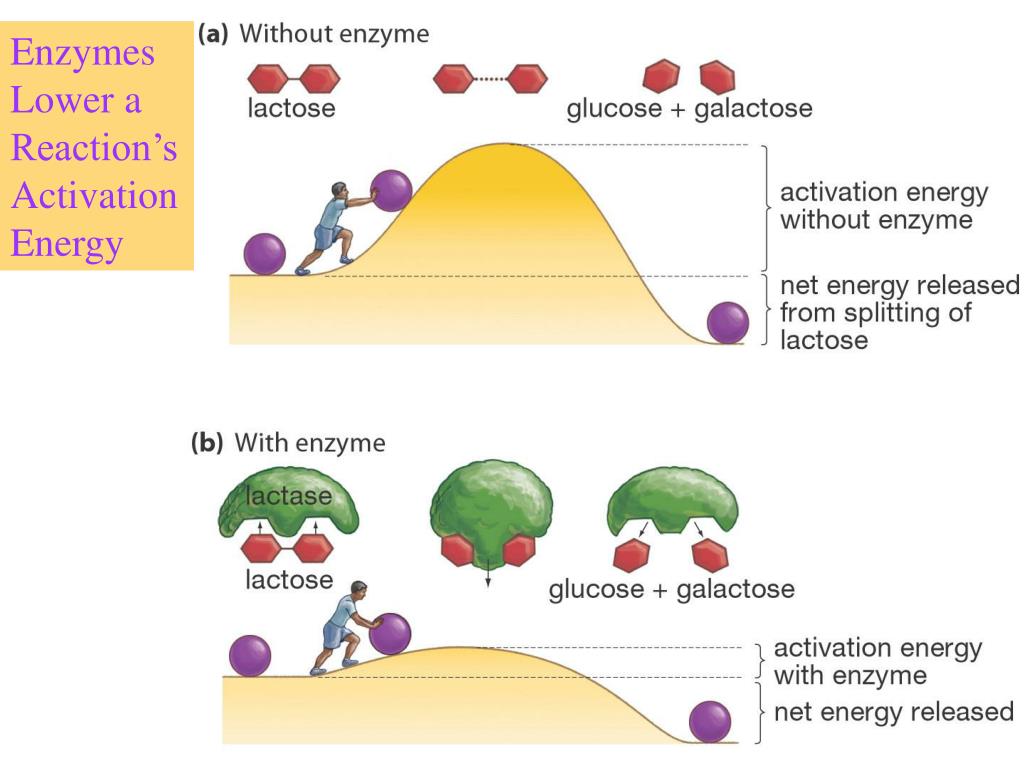
Unleashing The Power Of Enzymes How They Alter The Rules Of Chemical Reactions
The fundamental mechanism is substrate binding at an active site, where the enzyme stabilizes the transition state. This stabilization reduces the energy barrier between reactants and products. Without enzymes, most biological reactions would proceed far too slowly to sustain life. DNA replication alone would take years at uncatalyzed rates instead of minutes. The induced fit model describes how the active site changes shape when substrate binds. Early textbooks showed lock-and-key diagrams that implied rigid specificity. Real enzymes are more like flexible pockets that mold around their targets. This flexibility explains why some enzymes show promiscuity, processing multiple substrates with varying efficiency. Michaelis-Menten kinetics remains the standard framework for measuring enzyme activity. The Km value indicates substrate concentration at half-maximum velocity. Lower Km means higher apparent affinity, though this parameter depends heavily on experimental conditions. Temperature, pH, and ionic strength all shift the curve in ways that complicate direct comparisons between published values.
I encountered a particularly annoying edge case while optimizing a restriction digest for cloning work. The manufacturer's recommended buffer performed poorly with a methylated plasmid preparation. The enzyme was clearly active, as verified by control digestion of unmethylated DNA, but the specific substrate resisted cleavage despite extended incubation times. Adding bovine serum albumin at one hundred micrograms per milliliter resolved the inhibition. The supplier documentation mentioned BSA as a stabilizer but never noted its role in counteracting contaminant effects. I now include BSA as standard practice for any enzyme work involving crude DNA preparations. Allosteric regulation represents another layer of control that beginners often overlook. Enzymes with multiple subunits can exhibit cooperativity, where binding at one site affects activity at others. Hemoglobin demonstrates this principle, though it is technically not an enzyme. Aspartate transcarbamoylase shows classic allosteric behavior in pyrimidine biosynthesis, with CTP acting as an inhibitor and ATP as an activator. Catalytic efficiency combines turnover number with substrate affinity into a single metric. The kcat/Km ratio approaches the diffusion limit of approximately 10 to the eighth power per molar per second for ideal enzymes. Carbonic anhydrase and acetylcholinesterase operate near this theoretical ceiling. Most enzymes fall well below this maximum, which suggests evolutionary pressure favors adequate rather than optimal performance.
Get the Full Details

Enzyme inhibitors come in several mechanistic classes, each producing characteristic kinetic patterns. Competitive inhibitors increase apparent Km without affecting Vmax. Noncompetitive inhibitors decrease Vmax while leaving Km unchanged. Mixed inhibitors alter both parameters. Uncompetitive inhibitors reduce both Vmax and apparent Km proportionally. Lineweaver-Burk plots reveal these patterns through distinct line intersections, though modern researchers more commonly use nonlinear regression on raw velocity data. Practical enzyme handling requires attention to storage conditions that many protocols gloss over. Most enzymes lose activity gradually even under recommended storage temperatures. Aliquoting prevents degradation from repeated freezing and thawing. Some enzymes require reducing agents like DTT to maintain active site cysteines. Others aggregate in the presence of thiols. Testing storage conditions empirically often reveals discrepancies with published specifications. The industrial applications of enzymes extend far beyond molecular biology. Detergent proteases and lipases dominate household cleaning products. Amylases convert starch to sugar in brewing and baking. Lipases enable kinetic resolution of racemic mixtures in pharmaceutical synthesis. Immobilized enzymes allow continuous flow reactions that simplify purification and enable reuse.
Directed evolution has transformed enzyme engineering from rational design to selection-driven optimization. Frances Arnold received the Nobel Prize for developing this approach, which mimics natural selection in test tubes. Libraries of variant genes express enzymes with improved properties, and screening identifies useful variants. This method circumvents the incomplete understanding of enzyme structure-function relationships that limits purely computational design. Enzyme kinetics becomes challenging when substrate depletion, product inhibition, or enzyme instability confounds measurements. Initial rate conditions minimize these complications but require sufficient enzyme concentration to generate measurable signal within the linear time window. Conversely, too much enzyme depletes substrate too quickly for accurate measurement. Finding the right enzyme concentration involves trial and error even with well-characterized systems. I once attempted to measure the kinetics of a novel phosphatase using a coupled assay with NADPH monitoring. The observed rates decreased non-linearly over time, suggesting either enzyme instability or hidden complexity in the mechanism. Running the reaction without the coupling enzymes revealed that the phosphatase itself was inactivating with a half-life of approximately twenty minutes under assay conditions. The corrected kinetics showed standard Michaelis-Menten behavior once enzyme decay was accounted for. This experience taught me to always verify enzyme stability before interpreting kinetic data.
Modern structural biology provides atomic-level insights into enzyme mechanisms. X-ray crystallography captures static snapshots of enzyme-substrate complexes. Cryo-electron microscopy handles larger assemblies and conformational heterogeneity. Time-resolved crystallography and spectroscopy are beginning to capture reaction intermediates directly. Computational enzyme design remains a grand challenge despite recent advances. RosettaEnzyme and other platforms use energy scoring and sampling to propose active site mutations. Success rates remain modest, with useful improvements arising from a small fraction of designed variants. The fundamental difficulty lies in accurately modeling transition state energies and accounting for protein dynamics that contribute to catalysis. Enzyme engineering faces diminishing returns as improvements accumulate. The first round of directed evolution often produces dramatic gains. Subsequent rounds yield progressively smaller improvements as the enzyme approaches structural and mechanistic limits. Combining multiple beneficial mutations sometimes produces unexpected epistatic effects, where the combined phenotype differs from expectations based on individual variants.

Metabolic engineering relies heavily on enzyme optimization to redirect carbon flux through desired pathways. Overexpressing rate-limiting enzymes can increase product titers, but bottleneck shifting often reveals new limiting steps downstream. Balancing expression levels across multiple enzymes in a pathway requires tuning promoter strengths and copy numbers. The economic impact of industrial enzymes is substantial, measured in billions of dollars annually. Biocatalysis replaces harsh chemical conditions with aqueous environments at moderate temperatures and pressures. This reduction in energy consumption and waste generation aligns with green chemistry principles. Enzyme inhibition remains the primary mechanism of action for many pharmaceuticals. ACE inhibitors lower blood pressure by blocking angiotensin-converting enzyme. Protease inhibitors treat HIV by preventing viral polyprotein processing. Statins inhibit HMG-CoA reductase to reduce cholesterol synthesis. Understanding inhibition kinetics is essential for dose optimization and predicting drug interactions.
Some enzymes present unique handling challenges that deserve attention. Restriction enzymes from different suppliers show variable performance with the same substrate. Methylation-sensitive enzymes require specific DNA preparation methods. Polymerases differ in fidelity, processivity, and tolerance to modified nucleotides. Testing multiple sources and conditions often proves necessary before committing to a protocol. Enzyme assays vary enormously in complexity and throughput. Spectrophotometric assays monitor absorbance changes from NADH oxidation or phosphate release. Fluorometric assays offer greater sensitivity for low-activity enzymes. Coupled assays transfer product formation to an easily detectable reaction. High-throughput screening using microtiter plates enables rapid evaluation of variant libraries. The study of enzyme evolution reveals how new catalytic functions arise from existing protein scaffolds. Gene duplication followed by divergence creates paralogous enzymes with related but distinct specificities. Subfunctionalization divides ancestral functions between copies. Neofunctionalization creates entirely new activities through accumulated mutations.
Protein engineers face the challenge of balancing stability against activity. Mutations that improve thermostability often reduce catalytic efficiency. Rigidifying the active site can prevent the conformational changes required for catalysis. Finding mutations that improve both properties simultaneously remains difficult but achievable through careful screening. Enzyme immobilization on solid supports offers practical advantages for industrial applications. Support materials include agarose beads, silica particles, and magnetic nanoparticles. Covalent attachment, adsorption, and entrapment represent different immobilization strategies. Immobilized enzymes often show improved stability and can be reused multiple times, though mass transfer limitations may reduce apparent activity. The future of enzymology likely involves integration of computational and experimental approaches. Machine learning models trained on large enzyme sequence and activity databases may accelerate discovery. AlphaFold and related tools provide increasingly accurate structure predictions, though functional annotation remains challenging. Combining structure prediction with kinetic modeling could enable more rational enzyme engineering.

Workshop participants in enzyme characterization courses consistently underestimate the importance of proper controls. Including no-enzyme controls detects background activity from impurities. Substrate-only controls verify that signal arises from the expected reaction. Time-course measurements confirm linearity of initial rates. These simple checks prevent misinterpretation of data that would otherwise appear convincing.