How Photosynthesis Actually Works Under Real Conditions
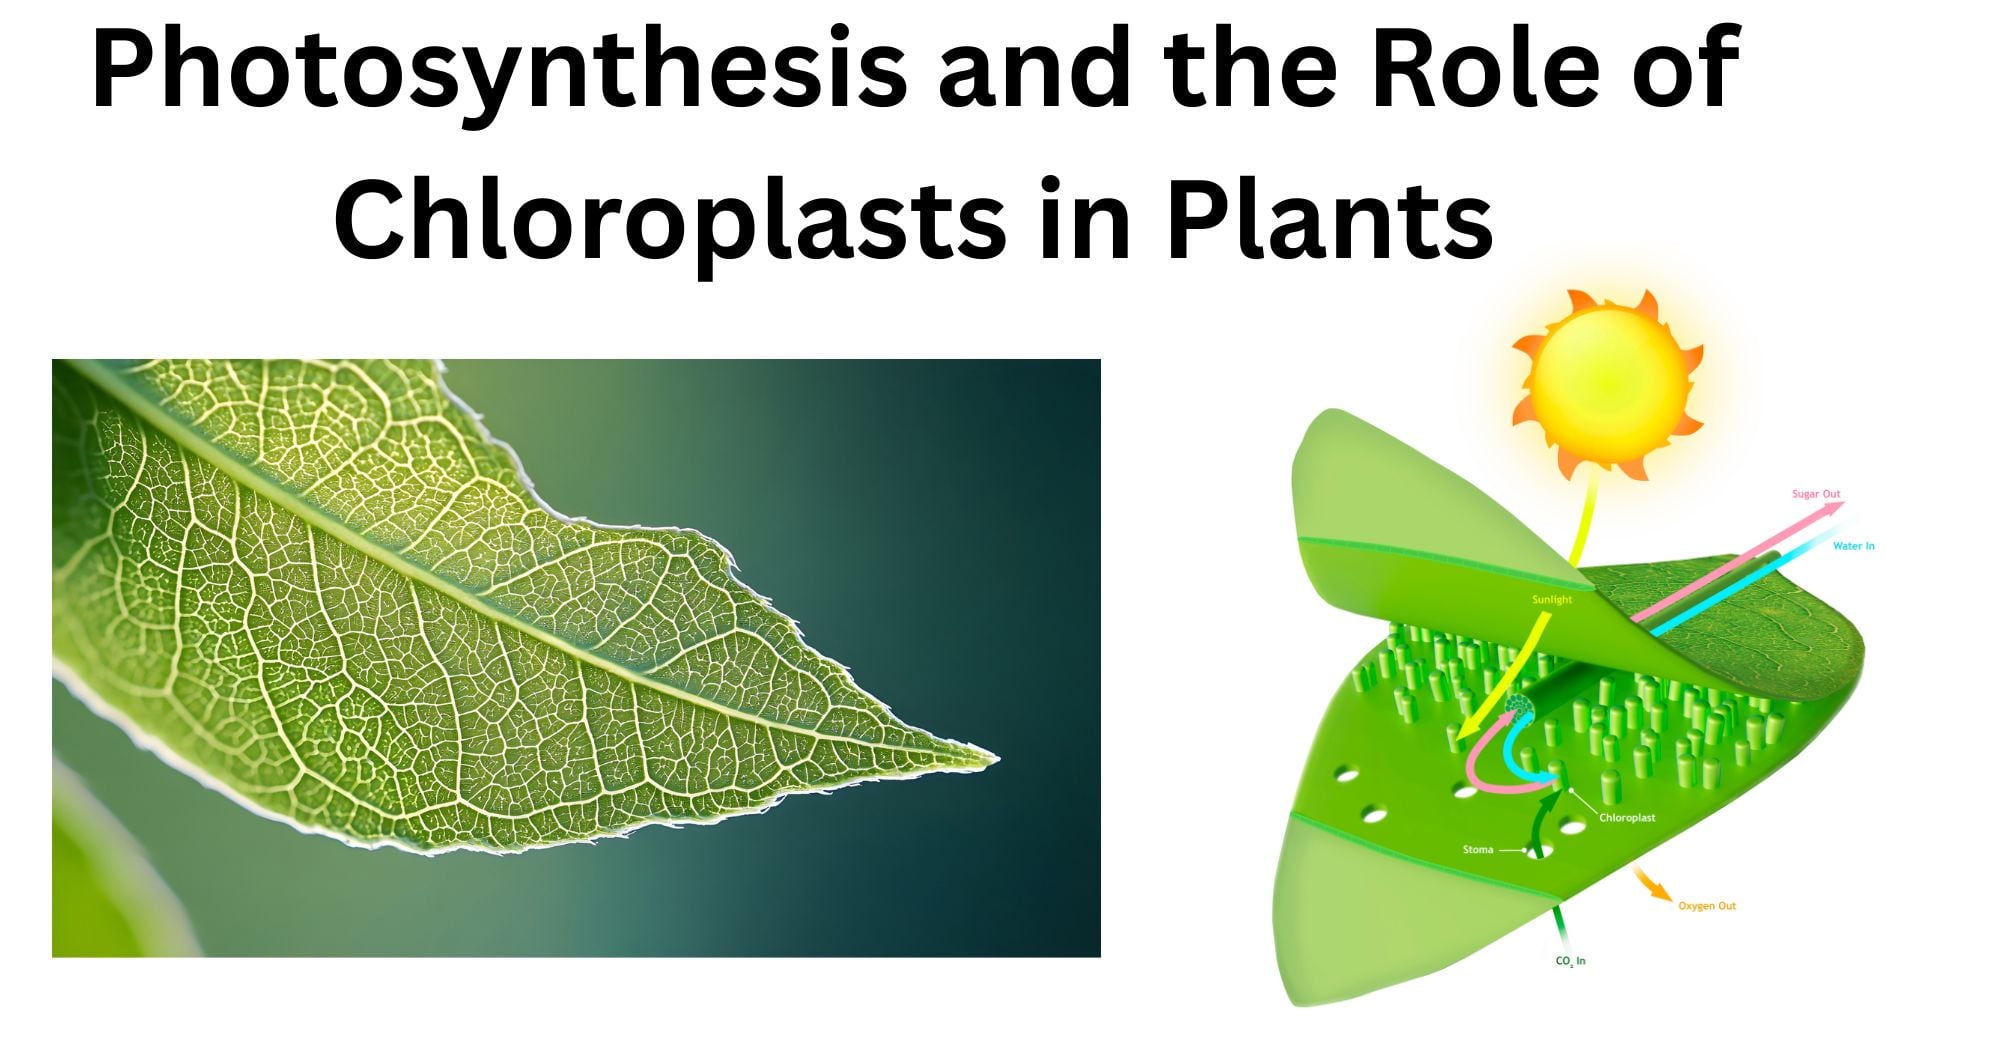
Most people think of chloroplasts as simple solar panels. They're not. They're dynamic, membrane-bound organelles with their own genome, double lipid bilayers, and a level of regulatory complexity that still trips up grad students in my lab. If you want to understand how a plant actually converts light into usable chemical energy, you have to look past the textbook diagram. I spent three summers measuring gas exchange and chlorophyll fluorescence on field-grown soybeans under heat stress. The data never matched the idealized models. Plants don't operate in controlled conditions. Light intensity shifts minute by minute, temperatures swing, CO2 availability at the leaf surface gets throttled by stomatal resistance you can't see. Understanding the fundamentals helps when things go sideways.Unleashing The Power Of Chloroplasts The Vital Role Of The Plants Primary Organelle
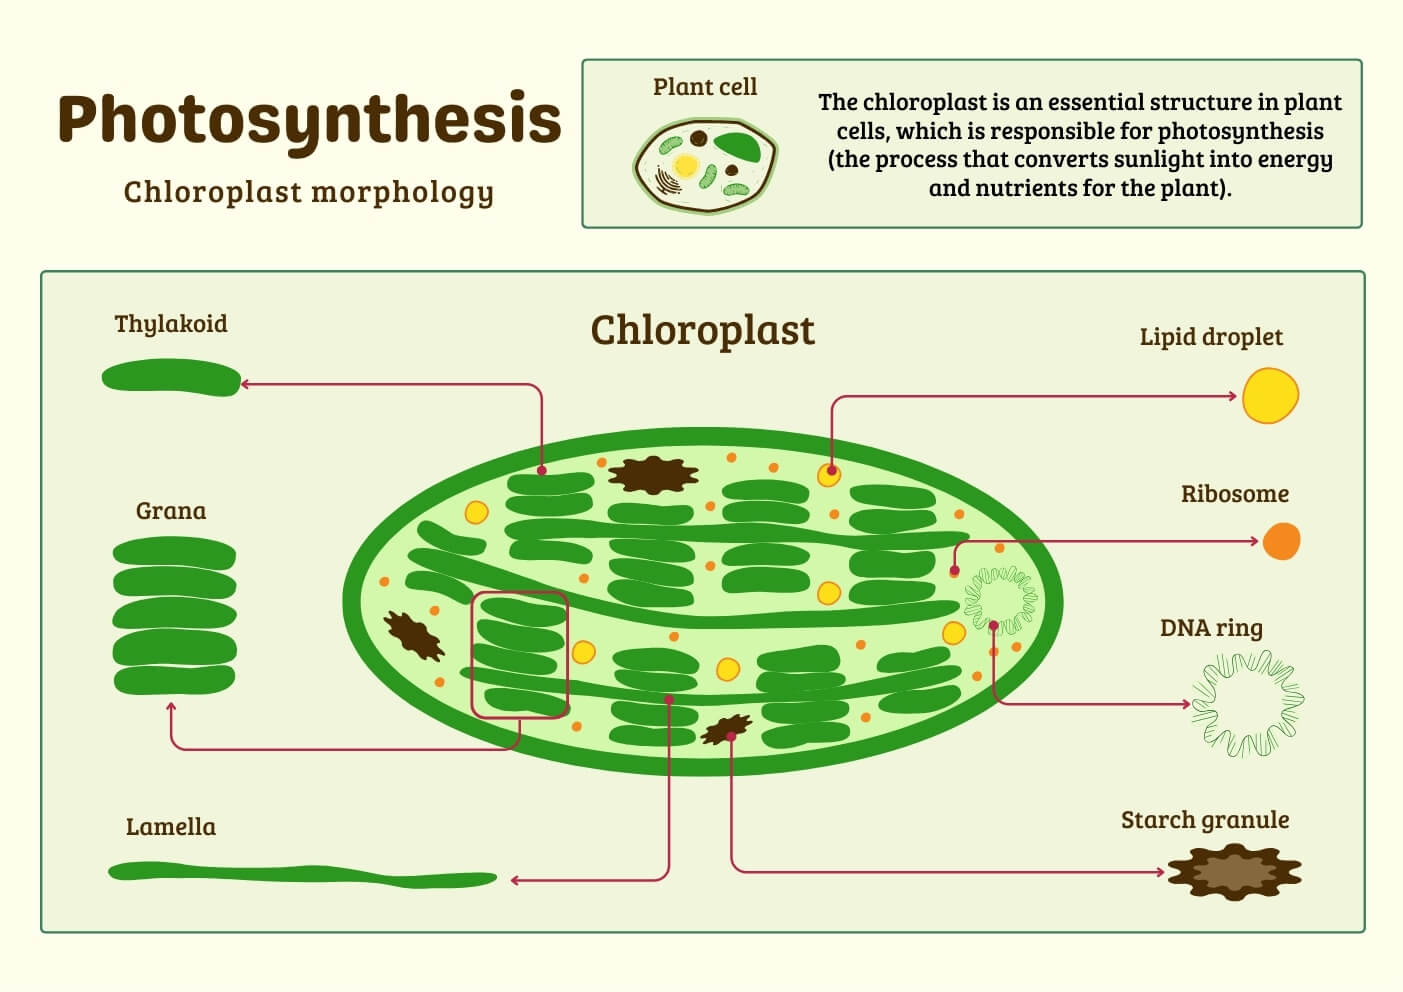
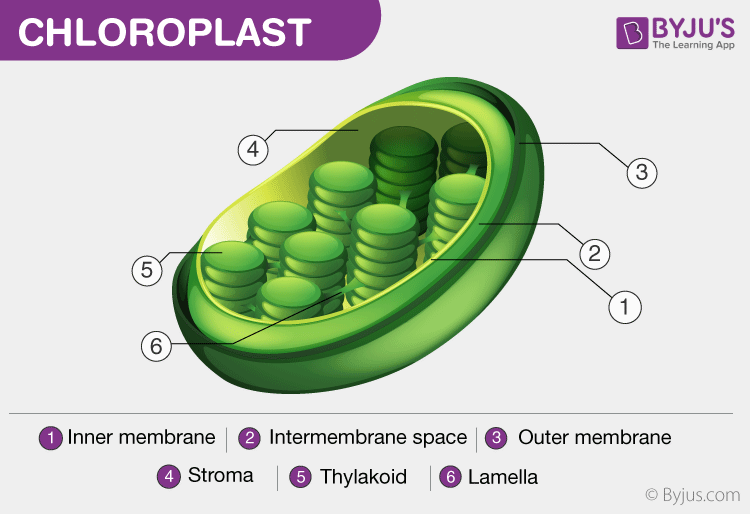
Chloroplasts contain two main functional compartments. The thylakoid membranes house the light-dependent reactions. Photosystem II splits water, generates a proton gradient, and passes electrons through plastoquinone, the cytochrome b6f complex, and plastocyanin to Photosystem I. That chain ends with ferredoxin and eventually NADP+ reductase producing NADPH. The proton gradient across the thylakoid membrane drives ATP synthase. That's roughly where introductory biology ends. The stroma is where the Calvin-Benson cycle operates. Rubisco fixes CO2 onto RuBP, producing two molecules of 3-phosphoglycerate. Most people don't realize that Rubisco is simultaneously a terrible enzyme. It has an oxygenase activity that triggers photorespiration, burning through energy instead of fixing carbon. Under normal atmospheric conditions, roughly 25 percent of Rubisco's catalytic events are oxygenations, not carboxylations. This is a massive efficiency loss built into the system.Photoprotection is non-negotiable. When light absorption exceeds what the Calvin cycle can process, excess energy damages the photosystems, particularly PSII. Plants use non-photochemical quenching (NPQ) through the xanthophyll cycle to safely dissipate that energy as heat. Violaxanthin converts to zeaxanthin under high light, and this process takes anywhere from seconds to minutes depending on the species and prior light history. If you're working with transient fluorescence measurements, ignoring NPQ kinetics will give you garbage data.
I once had a student try to run a pulse-amplitude-modulated fluorescence scan on cucumber leaves that had been kept in low light for two days, then moved directly into full sun for measurement. The Fv/Fm ratios came back at 0.32 instead of the expected 0.83 to 0.85 range. She assumed the equipment was broken. It wasn't. The plants were severely photoinhibited. We let them recover in dim light for four hours, and the ratios returned to normal. That's reversible damage, but repeated episodes compound. Chronic photoinhibition stunts growth significantly.The Structural Reality Inside a Chloroplast
Thylakoids aren't just floating membranes. They're organized into grana stacks connected by stroma lamellae. This architecture matters because it creates microenvironments. The lumen inside the grana becomes highly acidic during active photosynthesis, which is exactly what triggers NPQ through the PsbS protein. Stroma lamellae are richer in PSI and ATP synthase, while the grana cores concentrate PSII. This spatial separation isn't accidental. It optimizes electron flow and reduces wasteful short-circuiting. Chloroplasts divide by binary fission, inherited from their cyanobacterial ancestors. Each chloroplast contains between 20 and 100 copies of a circular DNA molecule, roughly 120 to 160 kilobases. Most of the original bacterial genes have migrated to the nuclear genome over evolutionary time. The chloroplast still encodes core photosynthetic proteins like D1 and D2 of PSII, the cytochrome b6f subunits, and RuBisCO large subunits. The nucleus encodes the rest, including virtually all the regulatory and assembly factors. This split-genome dependency is why chloroplast transformation in plants is so much harder than bacterial transformation. You're working with an organelle that depends on nuclear-encoded proteins imported through the TOC-TIC complexes in the outer and inner envelope membranes.C3, C4, and CAM: Different Strategies, Same Core Machinery
C3 plants run the standard Calvin cycle. Rubisco fixes CO2 directly in the mesophyll cells. This works fine in cool, moist environments but collapses under heat and drought because photorespiration accelerates faster than photosynthesis. C4 plants solved this with a spatial workaround. They use PEP carboxylase in mesophyll cells to fix CO2 into a four-carbon compound, then shuttle it into bundle sheath cells where Rubisco operates in a CO2-enriched environment. The cost is roughly 5 to 8 additional ATP per CO2 fixed, but the water-use efficiency and photosynthetic rate gains under hot conditions more than justify it. CAM plants take the same biochemistry but separate it temporally instead of spatially. They open stomata at night, fix CO2 into malate using PEP carboxylase, store it in the vacuole, and then release it during the day for the Calvin cycle. This is the most water-efficient strategy but the slowest in terms of growth rate. You'll see it in cacti, succulents, and many epiphytic orchids.I've personally encountered a situation where a researcher tried to extract intact chloroplasts from a C4 plant (sorghum) and ran a standard spinach chloroplast isolation protocol on it. The yield was abysmal and the preparations were non-photosynthetic. The issue was that sorghum bundle sheath chloroplasts are structurally different from mesophyll chloroplasts. They have reduced grana development and different envelope permeability. The sucrose gradient centrifugation parameters needed adjustment, and the homogenization buffer required a higher pH to keep those organelles from lysing. Nobody warns you about this in the methods section of a plant physiology textbook.