Monocotyledons are plants most people walk past every day without noticing the difference.
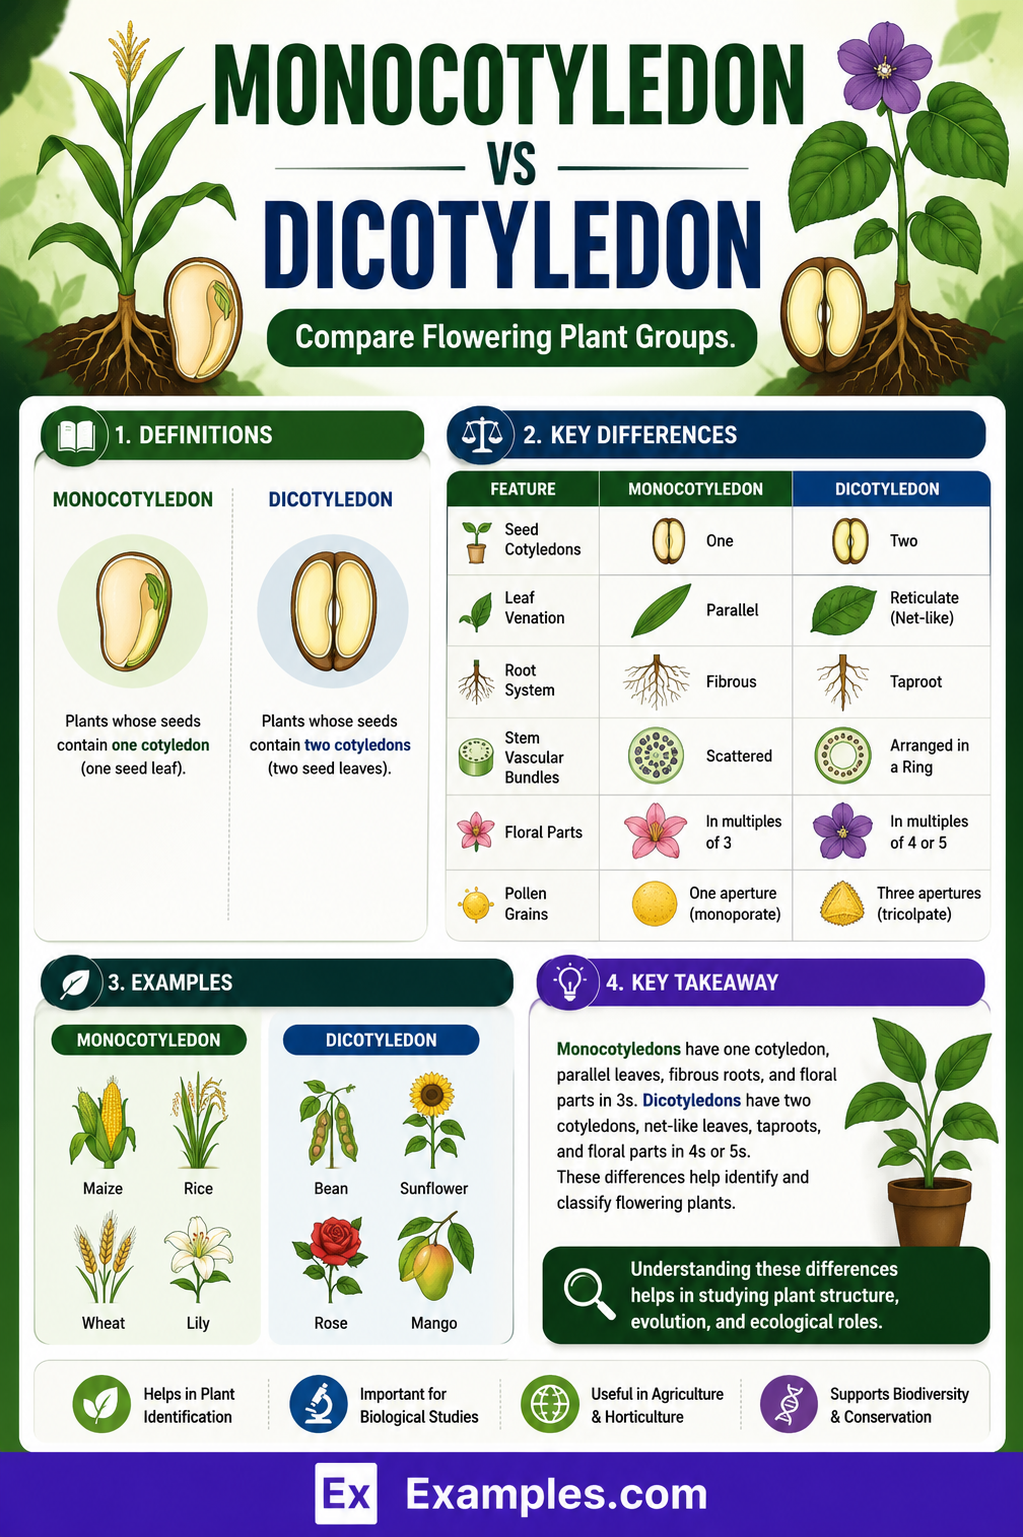
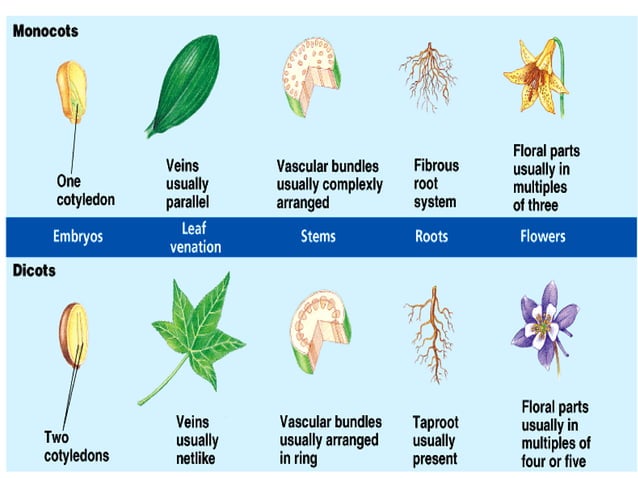
If you have ever tried to identify a plant and got told it is a monocot without understanding why that matters, you are not alone. The distinction is not just academic — it changes how the plant grows, how it responds to herbicides, and what root systems it will develop. I spent years getting tripped up by this because most introductory material presents monocots as a neat checklist. Real plants do not always follow the checklist. A monocotyledon, or monocot, is a flowering plant whose seed contains a single cotyledon. That one seed leaf is the starting point for everything else. From that single leaf, you get parallel vein patterns in the leaves, floral parts in multiples of three, scattered vascular bundles in the stem, and a fibrous root system rather than a taproot. These traits tend to co-occur because they share the same underlying developmental program. The way I approach identification is to start with the leaf veins. Parallel venation is the fastest field signal. If the veins run lengthwise without forming a net, it is almost certainly a monocot. I then check the stem cross-section if I am working with a cut sample. Scattered vascular bundles rather than a ring confirm it. Flower parts in threes seal the call.
I ran into a real problem a few years back when I was classifying a wetland plant that looked like a sedge but was growing in a habitat where sedges should not be dominant. The leaves had parallel veins and the stems were triangular, which pointed strongly toward Cyperaceae. But the floral anatomy was wrong for a typical sedge, and the vascular bundle arrangement in the stem did not match. I ended up dissectioning multiple specimens under a low-power scope and found that the perianth segments were actually reduced bracts, not true tepals. The plant was a member of Juncaceae, not Cyperaceae. The workaround was stopping reliance on external morphology alone and going straight to flower and fruit dissection, which removed the ambiguity entirely. It took about four hours per specimen instead of ten minutes, but it saved me from publishing the wrong classification.
Practical identification without the checklist trap
Most guides tell you to look for these five traits: single cotyledon, parallel veins, floral parts in threes, scattered vascular bundles, and fibrous roots. That is accurate on paper. In practice, exceptions show up constantly. Some monocots develop reticulate venation under certain conditions, and some have modified root systems that look more like taproots in early growth. Don't treat any single trait as definitive. The cotyledon itself is often overlooked because it only exists at germination. Once the seedling establishes, the cotyledon is either absorbed into the soil or becomes a temporary photosynthetic organ. If you are working with germinating seeds, preserving that first leaf is important. It is the only stage where you can directly observe the defining characteristic. I usually flatten and store germinated specimens in a press specifically for that reason. Vascular bundle arrangement is another trait that is easy to miss. You need a transverse stem section, stained if possible, viewed under magnification. The bundles appear as small dots scattered throughout the ground tissue rather than arranged in a circle. This is useful when leaf morphology is ambiguous, which happens frequently with grasses and related families that have highly modified leaves.
Get the Full Details
Major monocot families and what they look like in the field
The largest and most ecologically significant monocot families are Poaceae, Liliaceae, Orchidaceae, Arecaceae, and Iridaceae. Poaceae, the grass family, dominates many terrestrial ecosystems and includes virtually all major cereal crops. The leaves are alternate with sheathing bases, and the stems are hollow between nodes. Identification at the genus level within Poaceae often requires examining the inflorescence and glume structure, which is why field guides dedicated to grasses exist as separate volumes. Liliaceae contains many familiar garden plants and wild lilies. The flowers are typically showy with six tepals and six stamens. The leaves are basal or alternate with prominent arcuate veins. Orchidaceae is the other extreme — highly specialized flowers with fused reproductive structures and mycorrhizal dependence at germination. Many orchid seeds are dust-like and require fungal partners to complete development, which is why cultivating them from seed is significantly harder than most other monocots. Arecaceae, the palms, are trees and shrubs with unbranched stems and large crowns of leaves. The leaves are usually pinnate or palmate. Vascular bundles are scattered throughout the stem, and there is no true secondary growth. This means palms do not produce annual rings, and their stems increase in girth through primary growth and parenchyma expansion rather than cambial activity. That is a common misconception worth correcting early.
Counter-intuitive points most guides skip
One thing that catches people off guard is that monocots and eudicots are not a simple left-and-right division of the angiosperm world. The basal angiosperms and magnoliids occupy positions outside both groups. Plants like Amborella, water lilies, and magnolias share some monocot-like features but do not belong to the monocot clade. If you are building a phylogenetic framework, treating monocots as a monolithic group will distort your understanding of flowering plant evolution. Another overlooked point is that monocot flowers are not always in threes. While the ancestral condition is trimerous, many lineages have secondarily reduced or modified floral parts. Some grass flowers are highly reduced with minimal perianth, and some orchid flowers are so modified that counting parts becomes unreliable without careful dissection. The rule holds at the developmental level, but the adult morphology can be deceptive. Root system plasticity is also more common than textbooks suggest. Many monocots produce adventitious roots from the stem base, creating a dense fibrous mat. But in drought-prone environments, some species develop deeper anchor roots that functionally resemble taproots. If you are studying root architecture for agricultural purposes, assuming all monocots have shallow fibrous roots will lead to poor irrigation and anchoring decisions.
Herbicide sensitivity and practical implications
Monocots and eudicots respond very differently to many herbicides because of their distinct leaf anatomy and growth patterns. Broadleaf herbicides like 2,4-D target dicot growth patterns and are generally safe for turfgrasses, which are monocots. This is not because monocots are inherently resistant, but because the mechanism of action exploits differences in auxin transport and leaf venation architecture. Understanding this difference is critical for land management and avoids unnecessary damage to desirable plants. I once treated a lawn for weeds and accidentally oversprayed onto adjacent ornamental monocots. The damage was minimal compared to what would have happened to nearby eudicots. The practical takeaway is that monocot sensitivity to synthetic auxins is low, but not zero. Highly sensitive monocots like certain orchids and some monocot weeds can still be affected at elevated doses. Always calibrate application rates rather than assuming absolute safety.

Limitations of the monocot framework
The monocot category is useful but not universal. It does not explain everything about plant behavior or ecology. Mycorrhizal associations, for example, vary widely within monocots and cannot be predicted solely from classification. Some families form arbuscular mycorrhizae, while others, particularly many orchids, form ectomycorrhizae or rely on different fungal partners entirely. Using monocot status as a proxy for fungal association will produce incorrect conclusions. Similarly, the parallel vein rule breaks down in several well-documented cases. Some monocot leaves, particularly in early developmental stages or in specific genera, show reticulate or branched venation. If you encounter this, it does not mean the plant is a eudicot. It means the leaf is unusual, and you should verify with other characters rather than reclassifying based on one trait. Finally, monocot classification has undergone significant revision in recent decades. Molecular phylogenetics has reshaped family boundaries and relationships within the group. Older field guides may use outdated terminology or grouping that no longer reflects current understanding. When consulting references, check the publication date and prefer sources that incorporate APG IV systematics. The effort to verify takes minutes and prevents confusion later.
How to build a working identification workflow
Start with the leaf. Note venation pattern, leaf arrangement, and whether the leaf sheathes the stem. Move to the stem if accessible, checking for scattering vascular tissue or hollow internodes. Examine the flower structure if present, counting whorls and noting fusion. Check the fruit type, which can distinguish between closely related families. Document everything with photographs and measurements before disassembly. I usually take at least three photos per specimen: habit, leaf detail, and floral close-up. This prevents having to revisit the site for clarification. For seed-stage identification, preserve germinating specimens and label them immediately with collection data. Germination timing varies by species, and without labels, you will lose context within days. I keep a dedicated germination tray with waterproof tags and record ambient conditions alongside each specimen. The extra documentation step is about fifteen seconds per seed and prevents hours of confusion later.
When to use alternative approaches
Morphological identification reaches its limits with fragmentary material, highly modified specimens, or cryptic species complexes. In those cases, DNA barcoding using standard markers like rbcL, matK, and ITS provides reliable resolution. I recommend this approach when morphological characters are ambiguous after dissection and when accurate identification has ecological or management consequences. The cost per sample has dropped significantly, making it feasible for routine work rather than exceptional cases. If you are working with cultivated monocots where hybridization is common, morphological traits may be unreliable due to artificial selection. In those situations, cultivar records and propagation history are more trustworthy than field characteristics. I have seen specimens misidentified in horticultural databases because the original description was based on a confused cultivar name rather than verified morphology. Always trace nomenclature back to the publication when possible. Monocotyledons are straightforward once you stop treating them as a rigid set of rules and start treating them as a coherent developmental program with documented exceptions. The framework holds in the vast majority of cases. The edge cases are where the actual learning happens.

