The Chemical Exchange That Keeps Everything Alive
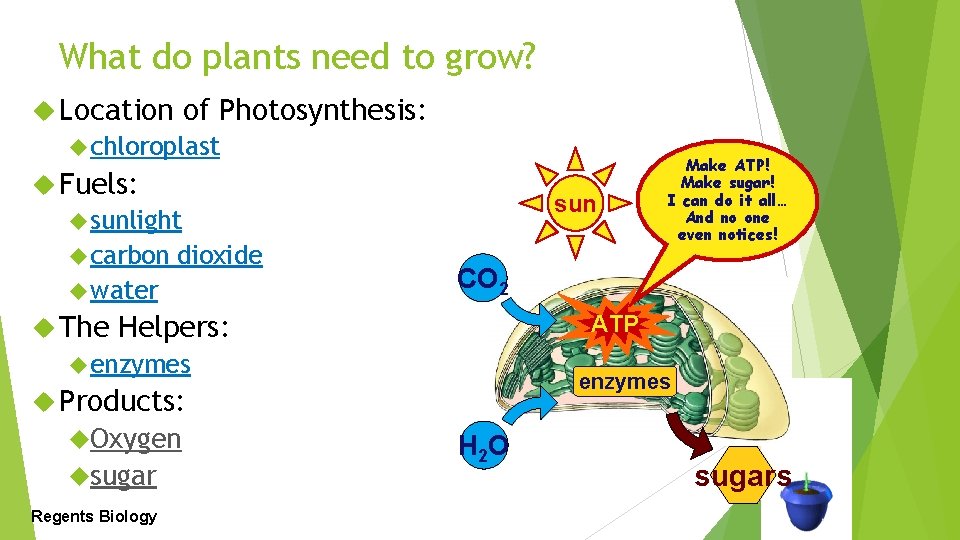
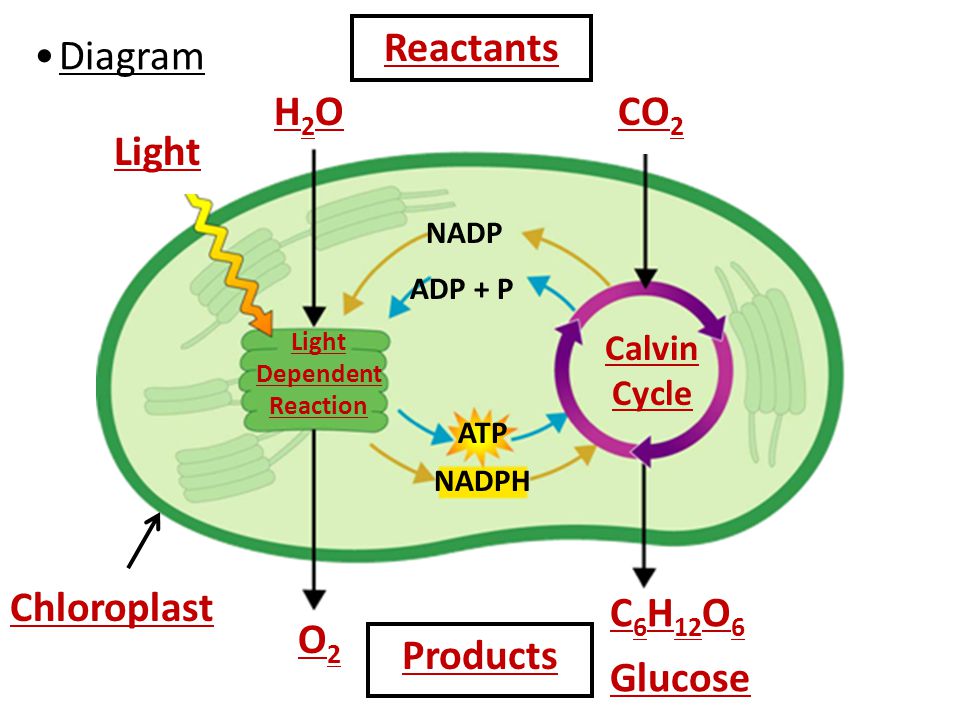
Plants take in carbon dioxide and water, convert sunlight into chemical energy, and release oxygen as a byproduct. This is photosynthesis, and it is the foundation of almost every food chain on Earth. The reactants are straightforward. Carbon dioxide enters through tiny pores called stomata. Water travels up from the roots through xylem tissue. Light energy is captured by chlorophyll molecules embedded in thylakoid membranes inside chloroplasts. The product side is equally simple on paper but messier in practice. Glucose forms as the primary energy storage molecule, though plants often convert it immediately into starch or sucrose for transport. Oxygen is released through those same stomata, creating the atmosphere we breathe. The balanced equation looks clean — six molecules of CO2 plus six molecules of H2O produce one glucose molecule, six molecules of O2, and energy stored in chemical bonds. Reality does not follow equations so neatly. I spent two summers studying photosynthetic rates in greenhouse-grown spinach varieties. The lab equipment recorded gas exchange using an infrared gas analyzer, and the data looked reasonable until I tried comparing leaf samples across different growth stages. Younger leaves with higher chlorophyll content per unit area showed dramatically different response curves than mature leaves, even when light intensity and CO2 concentrations were held constant. I initially attributed the variance to instrument drift, but running calibration checks showed the equipment was functioning correctly. The problem was biological. Photosynthetic capacity changes as leaves develop, and most standard protocols measure only fully expanded leaves without accounting for ontogenetic variation. Once I adjusted my sampling to include age-stratified measurements, the data became consistent. It took three weeks of rework to fix what looked like a simple experimental design error.
The light-dependent reactions occur in the thylakoid membranes and involve a series of electron transport chains that pump protons across the membrane, creating a gradient used by ATP synthase. This process generates ATP and NADPH, which then fuel the Calvin cycle in the stroma. The Calvin cycle fixes carbon dioxide into organic molecules through a series of enzyme-catalyzed reactions, with RuBisCO serving as the primary carbon-fixing enzyme. RuBisCO has a well-documented flaw. It can also catalyze a reaction with oxygen instead of carbon dioxide, initiating photorespiration, which wastes energy and reduces photosynthetic efficiency by up to twenty-five percent in C3 plants under hot, dry conditions. C4 and CAM plants evolved workarounds for this problem. Corn, sugarcane, and other C4 species spatially separate the initial carbon fixation from the Calvin cycle, concentrating CO2 around RuBisCO in bundle sheath cells. Succulents and cacti use temporal separation, opening stomata at night to fix CO2 into malate and releasing it during the day when photorespiration risk is lower. These adaptations matter when you are trying to optimize crop yields or understand plant responses to climate change. A C3 wheat field under elevated CO2 conditions might show fifteen to twenty percent yield increase, while a C4 maize field under the same conditions shows almost no response because maize is already operating near CO2 saturation. Oxygen production rates depend heavily on light quality, not just intensity. Blue and red wavelengths drive photosynthesis most efficiently, while green light penetrates deeper into the leaf mesophyll and contributes to overall rate in ways that simple quantum yield calculations do not capture. If you are growing plants under artificial light, full-spectrum LEDs that include both blue and red peaks will outperform single-wavelength sources, but the relationship between light quantity and photosynthetic output follows a saturation curve. Beyond a certain light intensity, increasing illumination provides diminishing returns because other factors become limiting, typically CO2 availability or enzyme reaction rates.
The glucose produced is rarely stored as free sugar. Plants convert it to starch for short-term storage within chloroplasts, to cellulose for structural purposes in cell walls, or to sucrose for transport through phloem to roots, fruits, and developing seeds. Understanding where the carbon ends up is crucial for agricultural applications. When you harvest a crop, you are removing stored photosynthetic products, and the plant must replenish those reserves through continued photosynthesis or mobilize reserves from other tissues. This is why defoliation during critical growth stages causes disproportionate yield losses compared to damage at other times. Temperature affects enzymatic reaction rates in the Calvin cycle, and the optimal range varies significantly between plant types. C3 plants typically peak around twenty to twenty-five degrees Celsius, while C4 plants operate optimally at twenty-five to thirty-five degrees. Above these ranges, enzyme denaturation and increased photorespiration reduce net photosynthetic rates. Below these ranges, reaction kinetics slow down, and in cold-adapted species, membrane fluidity changes can limit electron transport efficiency. This temperature dependency explains why tomato yields drop sharply during heat waves in greenhouse production, even when light and water are adequate. Water availability influences photosynthesis through stomatal regulation. When soil moisture drops below field capacity, plants close stomata to conserve water, which simultaneously blocks CO2 entry. The resulting decrease in intercellular CO2 concentration limits the Calvin cycle directly. However, prolonged drought causes additional damage through oxidative stress and potential chloroplast degradation. Irrigation management that maintains soil moisture between sixty and eighty percent of field capacity typically maximizes photosynthetic performance in most crops without wasting water on runoff or deep percolation.
Get the Full Details

CO2 enrichment represents one of the most reliable methods for boosting photosynthetic rates in controlled environments. Atmospheric CO2 sits around four hundred twenty parts per million, well below the saturation point for most C3 crops. Increasing concentration to one thousand to twelve hundred ppm can raise photosynthetic rates by thirty to fifty percent in lettuce, tomatoes, and cucumbers grown in greenhouses. This technique is standard practice in commercial horticulture but requires careful management of humidity and nutrient levels, since faster growth demands proportionally more water and minerals. Without adjusting fertilizer inputs, enriched CO2 environments can lead to nutrient deficiencies that mask the expected yield gains. Nutrient availability creates additional constraints. Nitrogen is a major component of chlorophyll and the enzymes involved in photosynthesis, including RuBisCO, which constitutes up to thirty percent of soluble leaf protein. Nitrogen deficiency manifests as chlorosis, reduced photosynthetic capacity, and lower biomass production. Magnesium forms the central atom in the chlorophyll molecule, and its deficiency produces interveinal chlorosis while directly impairing light capture. Phosphorus supports ATP formation and energy transfer, making it essential for both the light reactions and the Calvin cycle. Potassium regulates stomatal function and enzyme activation, linking water management to photosynthetic efficiency. Measuring photosynthesis accurately requires understanding what parameter you are actually recording. Net photosynthesis accounts for both carbon fixation and respiration, so it represents the difference between gross photosynthetic production and the CO2 released by mitochondrial respiration. On sunny days, the gap between net and gross photosynthesis can be substantial, particularly in C3 plants where photorespiration adds another layer of CO2 release. For most practical applications, net photosynthesis is the relevant metric because it reflects actual carbon gain available for growth and storage.
The relationship between photosynthesis and respiration shifts throughout the day and across seasons. During darkness, plants respire continuously, consuming oxygen and releasing CO2. At dawn, photosynthesis begins as light becomes available, and there is a compensation point where the rate of CO2 uptake equals the rate of CO2 release from respiration. Above this light compensation point, net photosynthesis becomes positive. The light compensation point varies between species and depends on temperature, CO2 concentration, and leaf nitrogen content. Shade-adapted species typically have lower compensation points because they invest less in photosynthetic machinery and respiration costs are reduced accordingly. Aging leaves undergo senescence, during which chlorophyll degrades and photosynthetic capacity declines. The nutrients from degraded proteins and chlorophyll are remobilized to younger tissues or storage organs, which is why older leaves turn yellow before they drop. This process is hormonally regulated, primarily through ethylene and abscisic acid signaling, and represents a strategic reallocation of resources rather than simply tissue failure. In perennial plants, this seasonal adjustment allows trees to survive winter by shedding leaves and conserving resources, while annual plants complete their lifecycle by allocating photosynthates to seed production before senescence. Stress responses complicate the picture further. Drought, salinity, extreme temperatures, pathogen attack, and herbivory all trigger physiological changes that alter photosynthetic performance. Some changes are immediate and reversible, like stomatal closure during water deficit. Others involve longer-term acclimation, such as adjustments in leaf orientation, cuticle thickness, or photosynthetic enzyme concentrations. Understanding whether a measured decrease in photosynthetic rate reflects acute stress or chronic adaptation requires knowing the timeline and severity of the stressor, as well as the species-specific response mechanisms at play.
For students and hobbyists interested in observing photosynthesis directly, the simplest demonstration involves aquatic plants like Elodea placed in inverted test tubes under bright light. Oxygen bubbles form on the plant surface and collect in the tube, providing visible evidence of O2 production. Adding sodium bicarbonate increases dissolved CO2 and typically accelerates bubble formation, demonstrating the CO2 limitation effect. However, this demonstration has limitations. Bubble counting is imprecise, temperature fluctuations affect gas solubility, and the relationship between bubble rate and actual photosynthetic rate is not linear. For more accurate measurements, dissolved oxygen probes or infrared gas analyzers are necessary, though those require equipment that most home labs do not have. Commercial applications of photosynthetic knowledge extend beyond agriculture into biotechnology and climate modeling. Engineering crops with improved RuBisCO specificity or introducing C4 photosynthetic pathways into C3 species remains an active area of research, with several transgenic approaches showing promise in field trials. Climate models incorporate photosynthetic parameters to predict vegetation responses to changing atmospheric composition, and uncertainties in these parameters represent a significant source of projection variance. The photosynthetic efficiency of global vegetation, measured as gross primary production, is estimated at approximately one hundred twenty to one hundred fifty petagrams of carbon per year, representing roughly thirty percent of the solar energy absorbed by land plants. Understanding the reactants and products of photosynthesis extends far beyond memorizing a chemical equation. It involves recognizing the complex regulatory networks, environmental dependencies, and evolutionary adaptations that determine how efficiently organisms convert light energy into usable chemical forms. The simplicity of the overall reaction masks decades of biochemical complexity, and appreciating that complexity is essential for anyone working in agriculture, ecology, or related fields. The oxygen you inhale right now was produced by photosynthetic organisms, likely within the last few seconds to minutes, cycling through an process that has operated continuously for over three billion years.