What Actually Happens When You Map Food Webs
I used to think trophic relationships were just chains — grass eats sun, deer eats grass, wolf eats deer. Simple enough for a high school biology diagram. Then I spent three field seasons in a coastal estuary trying to track energy flow through a system where everything ate everything else, and the real structure became painfully obvious. It is not a grid of individual relationships. It is a single continuous energy transfer network.Trophic Relationships Definition The Hidden Power Grid That Keeps Ecosystems Alive
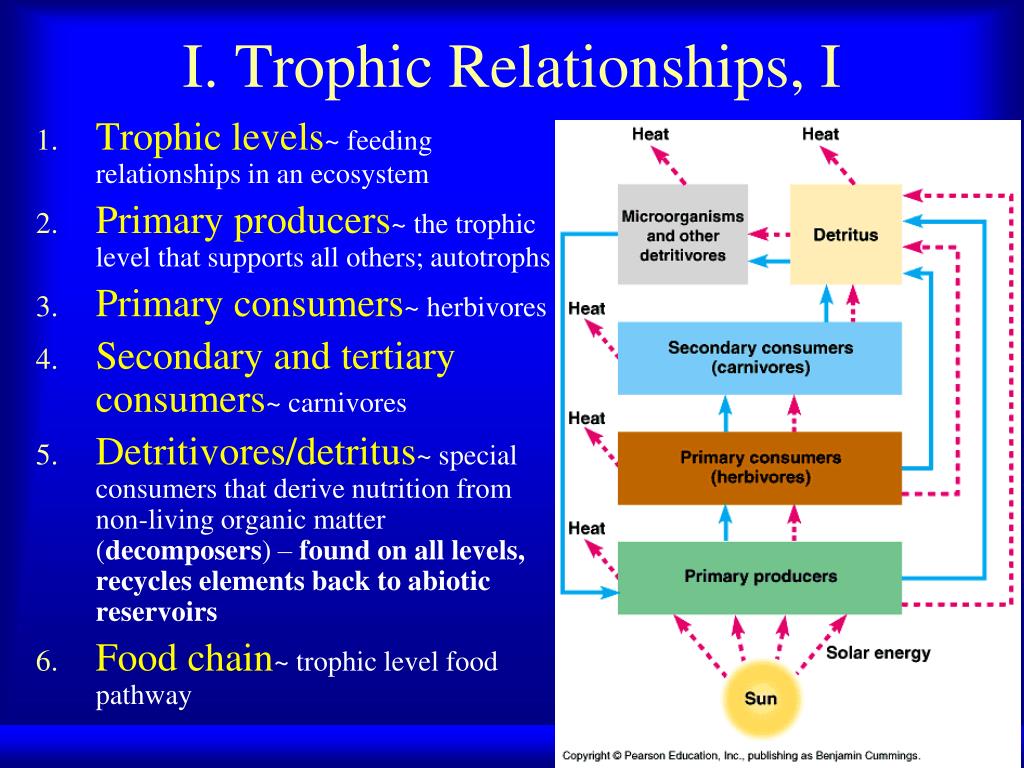
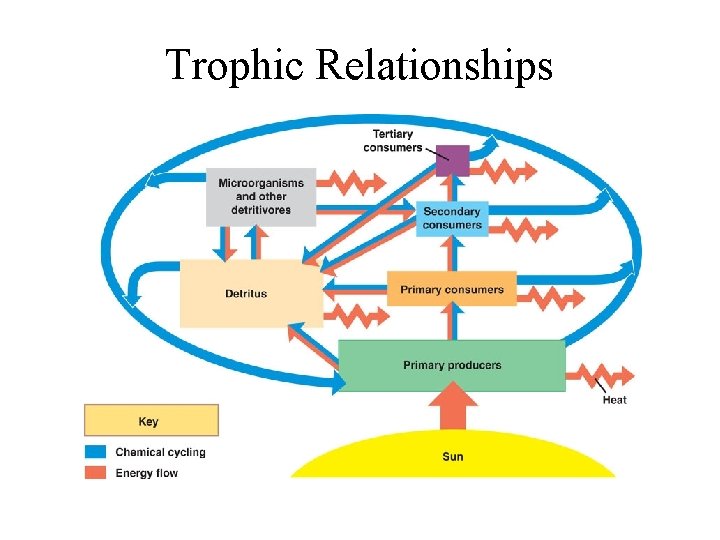
A trophic relationship describes how energy and nutrients move from one organism to another through feeding interactions. Each organism occupies a position called a trophic level. Primary producers — plants, algae, photosynthetic bacteria — capture solar or chemical energy and convert it into biomass. Primary consumers eat the producers. Secondary consumers eat the primary consumers. Tertiary and quaternary consumers occupy the top positions in most food chains. The key term here is transfer efficiency. Only about 10 percent of energy at one trophic level makes it to the next. The rest is lost as heat through respiration, excreted as waste, or simply passed through undigested. This 10 percent rule is not a hard law. It varies between 5 and 20 percent depending on the ecosystem, but the pattern is consistent everywhere. I remember spending two weeks in 2019 trying to reconcile biomass data from a marsh system with textbook energy pyramid diagrams. The numbers did not add up. The decomposers — fungi, bacteria, detritivores — were consuming far more energy than the direct herbivory path explained. That was when I stopped thinking in straight chains and started thinking in networks. The hidden architecture is the detrital pathway, and it carries more energy than the grazing pathway in most terrestrial ecosystems.
Energy Flow Is the Real Mechanism
People focus on who eats whom. That is the visible part. The invisible part is energy. Every trophic interaction is fundamentally an energy transaction. When a largemouth bass consumes a bluegill, it is acquiring approximately 10 percent of the energy the bluegill had stored. The bass then uses most of that remaining energy for metabolism, movement, and thermoregulation. Only a small fraction becomes new bass tissue available to the next consumer. This energy constraint determines everything about ecosystem structure. It limits how many trophic levels exist. Most ecosystems have four or five. Beyond that, there is simply not enough energy to sustain another level. A sixth level would require an energy input that no practical ecosystem can provide. Some aquatic systems with extremely efficient phytoplankton production reach six, but those are rare exceptions. I worked with a graduate student once who was modeling carbon flow through a temperate forest. Her initial model assumed a simple linear chain: leaves to caterpillars to birds to hawks. The system kept collapsing because she could not get enough energy to reach the hawks. We spent a month tracking down the missing pathway. It turned out the majority of leaf biomass never went through caterpillars. It went through detritus — fallen leaves decomposed by fungi and bacteria, consumed by soil invertebrates, which then fed the birds. The model only worked when we added the detrital loop.
Trophic Levels Are Not Clean Categories
The textbook diagram shows discrete levels. Reality does not work that way. Most consumers occupy multiple trophic positions. A raccoon eats berries (primary consumer) and crayfish (secondary consumer). A bear eats salmon (tertiary consumer) and roots (primary consumer). Omnivory is the default state, not the exception. When you calculate a species actual trophic position, you use stable isotope analysis. Nitrogen-15 ratios increase predictably with each trophic step. A plant might register at 3.5 ‰ above atmospheric nitrogen. A herbivore eating that plant sits at 6 to 7 ‰. A predator eating the herbivore sits at 9 to 10 ‰. But individual variation means a single animal might show a value between levels. That is normal. I had an ecologist colleague who spent four years studying a single fish species in a lake system. She expected to place it cleanly at trophic level 3.5 based on stomach content analysis. The isotope data placed it at 4.1. The discrepancy came from cannibalism — the fish were eating their own young, which pushed them up a half level. If you only looked at what they ate during the day, you would miss the nocturnal predation entirely. Stomach contents give you a snapshot. Isotopes give you a months-long average. Use both.
Get the Full Details

The Structural Role of Top Predators
Top predators regulate energy distribution across the entire network. Remove them and the system reorganizes. This is the trophic cascade effect. The classic example is wolves in Yellowstone, but the mechanism applies everywhere from sea otters to sharks to spiders. When a top predator disappears, mesopredators — mid-level carnivores — increase in abundance. They overconsume their prey, which reduces the prey population, which releases the prey's food source from consumption pressure. The cascade moves down through multiple levels. In the Yellowstone case, elk overbrowsed willow and aspen along rivers. After wolf reintroduction, riparian vegetation recovered. Beavers returned. The physical habitat changed. I worked on a project in the Pacific Northwest studying the effects of orca population decline on marine food webs. Killer whales had shifted from hunting seals and sea lions to focusing on smaller prey, including dolphins and porpoises. The mid-level predator release created unexpected pressure on fish populations. The data showed a clear correlation between orca foraging shift and declining herring biomass. It was not a simple top-down control anymore. The energy flow pathways had rerouted through unfamiliar connections.
Detritus Is Not Dead Energy
Decomposition is where most trophic energy actually flows. In many ecosystems, up to 90 percent of primary production enters the food web as dead material rather than through direct herbivory. Fungi and bacteria break down complex molecules — lignin, cellulose, chitin — that most animals cannot digest. The nutrients released become available to primary producers, closing the loop. This detrital pathway operates independently of the grazing pathway. It has its own set of organisms, its own energy efficiencies, and its own vulnerabilities. Pesticides, heavy metals, and microplastics accumulate through this pathway just as they do through grazing chains. The difference is timing. Detrital organisms process material slower, so contaminants persist longer in soil and sediment food webs. During a wetland restoration project in Louisiana, I observed this firsthand. We planted cordgrass and expected rapid establishment. It did not happen. The soil microbiome had been disrupted by previous oil contamination. Decomposer populations were depressed. Without active decomposition, nutrient cycling stalled. The plants starved despite adequate light and water. We added substrate from an uncontaminated nearby site to inoculate the soil with functional decomposer communities. Establishment improved within two growing seasons.
Human Impact Is a Structural Problem
Habitat destruction, overharvesting, and invasive species do not just reduce species counts. They restructure energy flow pathways. When a keystone species is removed, the entire network reorganizes. Some pathways collapse. Others emerge. The total energy flow through the system usually decreases because simplified networks are less efficient at capturing and retaining energy. Fishing is the clearest example. Industrial trawling removes biomass faster than trophic replacement can occur. When large predators are depleted, the system shifts toward smaller, faster-reproducing species. The total catch might remain stable, but the energy throughput changes. You are harvesting different parts of the network with different efficiencies. The caloric yield per unit of primary production drops significantly. I consulted on a fishery management plan in the Gulf of Mexico where the data showed consistent declines in trophic level of the catch over two decades. This is the fishing-down-the-food-web phenomenon. The system was being stripped of higher trophic species, leaving lower-level organisms. Energy flow through the remaining web was less stable, more variable, and more susceptible to environmental fluctuations. The plan recommended reducing fishing mortality on mid-trophic species to allow recovery of the full network structure.

Measuring Trophic Networks Requires Multiple Approaches
Stomach content analysis gives you direct feeding evidence but only captures recent meals. Stable isotope analysis gives you integrated dietary information over weeks or months. Both have blind spots. DNA metabarcoding of gut contents or feces has become standard in recent years. It identifies prey species from trace DNA, catching items that stomach dissection misses entirely. The combination of these methods reveals network complexity that any single approach obscures. A 2022 study of a tropical reef system used all three techniques simultaneously. Stomach content analysis identified 47 prey species. Isotope analysis suggested 12 trophic positions. DNA metabarcoding identified 134 prey species, 87 of which were missed by the other methods. The trophic network had twice as many links as previously documented. This matters for conservation. If you model a food web with incomplete link data, you underestimate resilience. Real networks with more connections distribute energy loss differently. They absorb perturbations through alternative pathways. Models built on partial data predict catastrophic collapse where the actual system might reorganize and persist.
Common Misunderstandings
People often treat trophic levels as fixed categories. They are not. An organism's trophic position varies with life stage, season, and location. A frog eating insects as a tadpole occupies a different trophic level than the same frog eating insects as an adult, because the insect prey community differs. Larval and adult stages often occupy distinct niches within the same network. Another misconception is that energy flow equals population size. It does not. A system can have enormous primary producer biomass but low consumer biomass if turnover rates differ. Phytoplankton reproduce rapidly. Zooplankton consume them continuously. The standing stock of phytoplankton at any moment is smaller than the zooplankton eating it, but the energy flow supports the larger biomass through rapid replacement. I spent a semester teaching ecology and noticed students consistently confused biomass pyramids with energy flow. They assumed a pyramid shape meant more energy was available at each level. The pyramid shape reflects mass accumulation, not energy transfer rate. An inverted pyramid of biomass can exist when primary producers have high turnover. The energy flow still moves upward, diminishing at each level, regardless of biomass arrangement.
Why This Matters Practically
Understanding trophic relationships is essential for ecosystem management. Every intervention — stocking, removal, habitat modification — affects energy flow. Restoring a wetland requires rebuilding the full trophic network, not just planting vegetation. Reintroducing a predator requires assessing whether the prey base and intermediate consumers can support it. Fishing quotas should account for trophic position, not just species identity. The energy transfer framework also explains why some interventions fail. Adding nutrients to a lake increases primary production. That should benefit everything up the chain. But if the system lacks the consumer groups needed to process the extra biomass, the nutrients accumulate as algal blooms rather than flowing through productive food webs. The trophic structure was missing the connectors. The energy had nowhere to go. I worked with a restoration team in Chesapeake Bay that added oyster larvae to a degraded reef. The larvae settled successfully. The reef grew. But the expected increase in filter-feeding and subsequent energy redistribution did not materialize for three years. The problem was sediment composition. The larvae settled on unstable substrate that shifted with tidal flow. By the time the reef stabilized, the local food web had reorganized around different species. The oysters were present but functionally replaced in the trophic network.

The Bottom Line
Trophic relationships are not simple chains. They are dynamic energy networks where most flow occurs through detrital pathways, where organisms occupy multiple positions, and where structural changes propagate through the entire system. The 10 percent energy transfer rule constrains everything. The complexity of real networks exceeds textbook models. Management and conservation require understanding the full network structure, not just the visible feeding relationships. The practical takeaway is that ecosystem integrity depends on complete trophic structure. Removing any component — predator, prey, decomposer — alters energy flow patterns throughout the system. Restoration must rebuild those connections. Monitoring must track energy pathways, not just species counts. The hidden power grid is what sustains the visible life.