Light, Water, and Carbon Dioxide: The Mechanical Reality
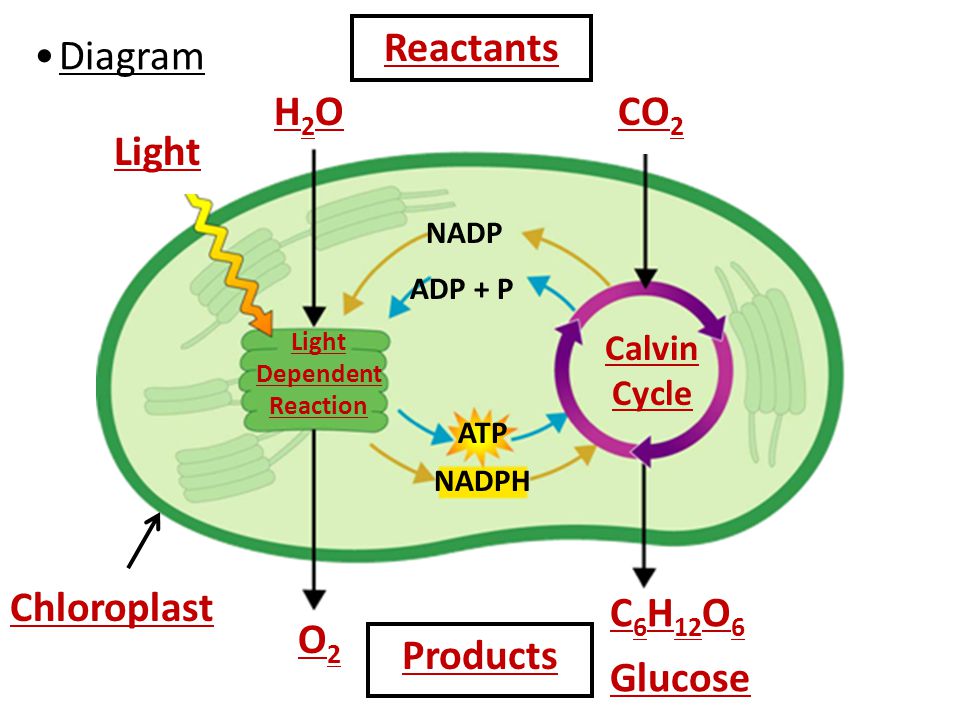
Photosynthesis is not some mystical natural process. It is a series of chemical conversions that any biology student will need to understand for exams, teaching certifications, or just getting through introductory botany. The core equation is standard material. Six molecules of carbon dioxide and six molecules of water, in the presence of light energy, produce one molecule of glucose and six molecules of oxygen. That is the simplified textbook version. The actual mechanism inside a chloroplast is considerably messier. The reactants enter through two separate pathways. Carbon dioxide diffuses into the leaf through stomata, tiny pores on the underside of most plant leaves. Water travels upward from the roots through xylem tissue, pulled along by transpiration. These two substances never really meet until they are inside the chloroplast stroma, and even then their timing matters. Light absorption happens in the thylakoid membranes, where chlorophyll and accessory pigments capture photons. The energy from those photons drives the splitting of water molecules, a process called photolysis. This releases electrons, protons, and oxygen as a byproduct. The oxygen exits the leaf and eventually reaches your lungs.
The Vital Cycle Of Life Understanding Reactants And Products Of Photosynthesis
When you actually work with this material, the confusion usually comes from treating the light-dependent and light-independent reactions as if they operate independently. They do not. The Calvin cycle, which fixes carbon dioxide into glucose, requires ATP and NADPH produced during the light reactions. Without a steady supply of those energy carriers, carbon fixation grinds to a halt within seconds. I remember running a school lab where students measured oxygen production under different light intensities using aquatic plants like Elodea. We expected a clean linear relationship between light intensity and oxygen output. Instead, the data flattened out completely beyond a certain threshold. The light reactions were saturated. The Calvin cycle enzymes, particularly RuBisCO, were operating at maximum capacity and could not process the incoming ATP and NADPH any faster. More light was literally useless. The limiting factor had shifted from light to enzyme concentration and carbon dioxide availability. This is the practical takeaway that most study guides miss. The rate of photosynthesis is never controlled by just one variable. You have light intensity, carbon dioxide concentration, temperature, water availability, and the concentration of photosynthetic enzymes all interacting simultaneously. Change one and the others become more or less relevant. A C3 plant in a hot dry environment will close its stomata to conserve water, which cuts off its carbon dioxide supply. Photosynthesis drops, not because there is no light, but because the plant traded carbon intake for water retention. This is a routine tradeoff that plants make constantly. There is also the matter of photorespiration, which is essentially RuBisCO making a mistake. The enzyme is supposed to attach carbon dioxide to a five-carbon sugar called RuBP. But sometimes it attaches oxygen instead. This produces a useless two-carbon compound that the plant has to recycle through an expensive metabolic pathway called the photorespiratory carbon oxidation cycle. Photorespiration can drain up to fifty percent of the fixed carbon in C3 plants under warm conditions. C4 plants solved this problem evolutionarily by separating the initial carbon fixation from the Calvin cycle spatially. They use a different enzyme, PEP carboxylase, in mesophyll cells to fix carbon into a four-carbon compound, then shuttle that compound into bundle sheath cells where the Calvin cycle runs at higher carbon dioxide concentrations. CAM plants take the same biochemical solution but separate it temporally, opening their stomata at night to fix carbon and running the Calvin cycle during the day. These adaptations matter enormously if you are working with crops or trying to understand why certain plants dominate in specific environments.
What Actually Comes Out
The products of photosynthesis are glucose and oxygen, but calling glucose the main product oversimplifies things. Plants convert the initial glucose into starch for storage, cellulose for cell walls, and a wide variety of other organic compounds. The glucose molecule itself is a starting point, not an endpoint. Oxygen, on the other hand, is largely a waste product from the plant's perspective. The plant does not use the oxygen it produces for respiration in any significant way during daylight. Most of it diffuses back out through the stomata. This is why forests and phytoplankton are critical to atmospheric composition, not because plants need the oxygen they release, but because everything else on Earth does. If you are preparing teaching materials or studying for an exam, focus on the stoichiometry. The molar ratio of carbon dioxide consumed to oxygen produced is one to one. One molecule of CO2 in, one molecule of O2 out, for each turn of the cycle. It takes six turns to produce one glucose molecule. The ATP and NADPH consumed in the Calvin cycle are regenerated in the light reactions. If a question asks how many ATP and NADPH molecules are required to fix six carbon dioxide molecules, the answer is eighteen ATP and twelve NADPH. Memorizing that number will save you time on multiple choice sections. One limitation worth noting is that photosynthesis as taught in introductory courses describes a theoretical maximum. Real plants operate well below that maximum due to environmental stress, pathogen damage, nutrient deficiency, and the inherent inefficiency of RuBisCO. Net primary productivity in most terrestrial ecosystems is roughly one to two percent of the solar energy that reaches the vegetation. The rest is reflected, transmitted, or lost as heat. Agricultural crops are slightly more efficient but still far below the theoretical limit. If someone presents photosynthesis as a highly efficient energy conversion process, they are describing the biochemistry in isolation, not the biological reality.
Get the Full Details

Practical Considerations
Measuring photosynthetic rate in a lab or field setting requires deciding what proxy you are tracking. Oxygen production is the most direct measure of the light reactions. Carbon dioxide uptake reflects the Calvin cycle. Biomass accumulation is the slowest but most comprehensive indicator. Each method has blind spots. Dissolved oxygen sensors drift over time and require regular calibration. Infrared gas analyzers for CO2 measurement are accurate but expensive and sensitive to ambient humidity. Dry biomass measurement destroys the sample and requires weeks of growth time. I prefer measuring oxygen evolution in aquatic plants when possible. It is cheap, relatively straightforward, and the results are immediately visible. Terrestrial leaf disc assays work too, though they take longer to set up and the floating disk method introduces variability based on leaf thickness and air content in the spongy mesophyll. The bottom line is that photosynthesis is a constrained chemical process, not an infinite energy source. The reactants must arrive at the right place at the right time, the enzymes must be functional, and the environmental conditions must stay within a range that does not denature proteins or close stomata. Understanding what limits the process in any given situation is more useful than memorizing the balanced equation.