Cellular Respiration and Why the Mitochondrion Gets All the Credit
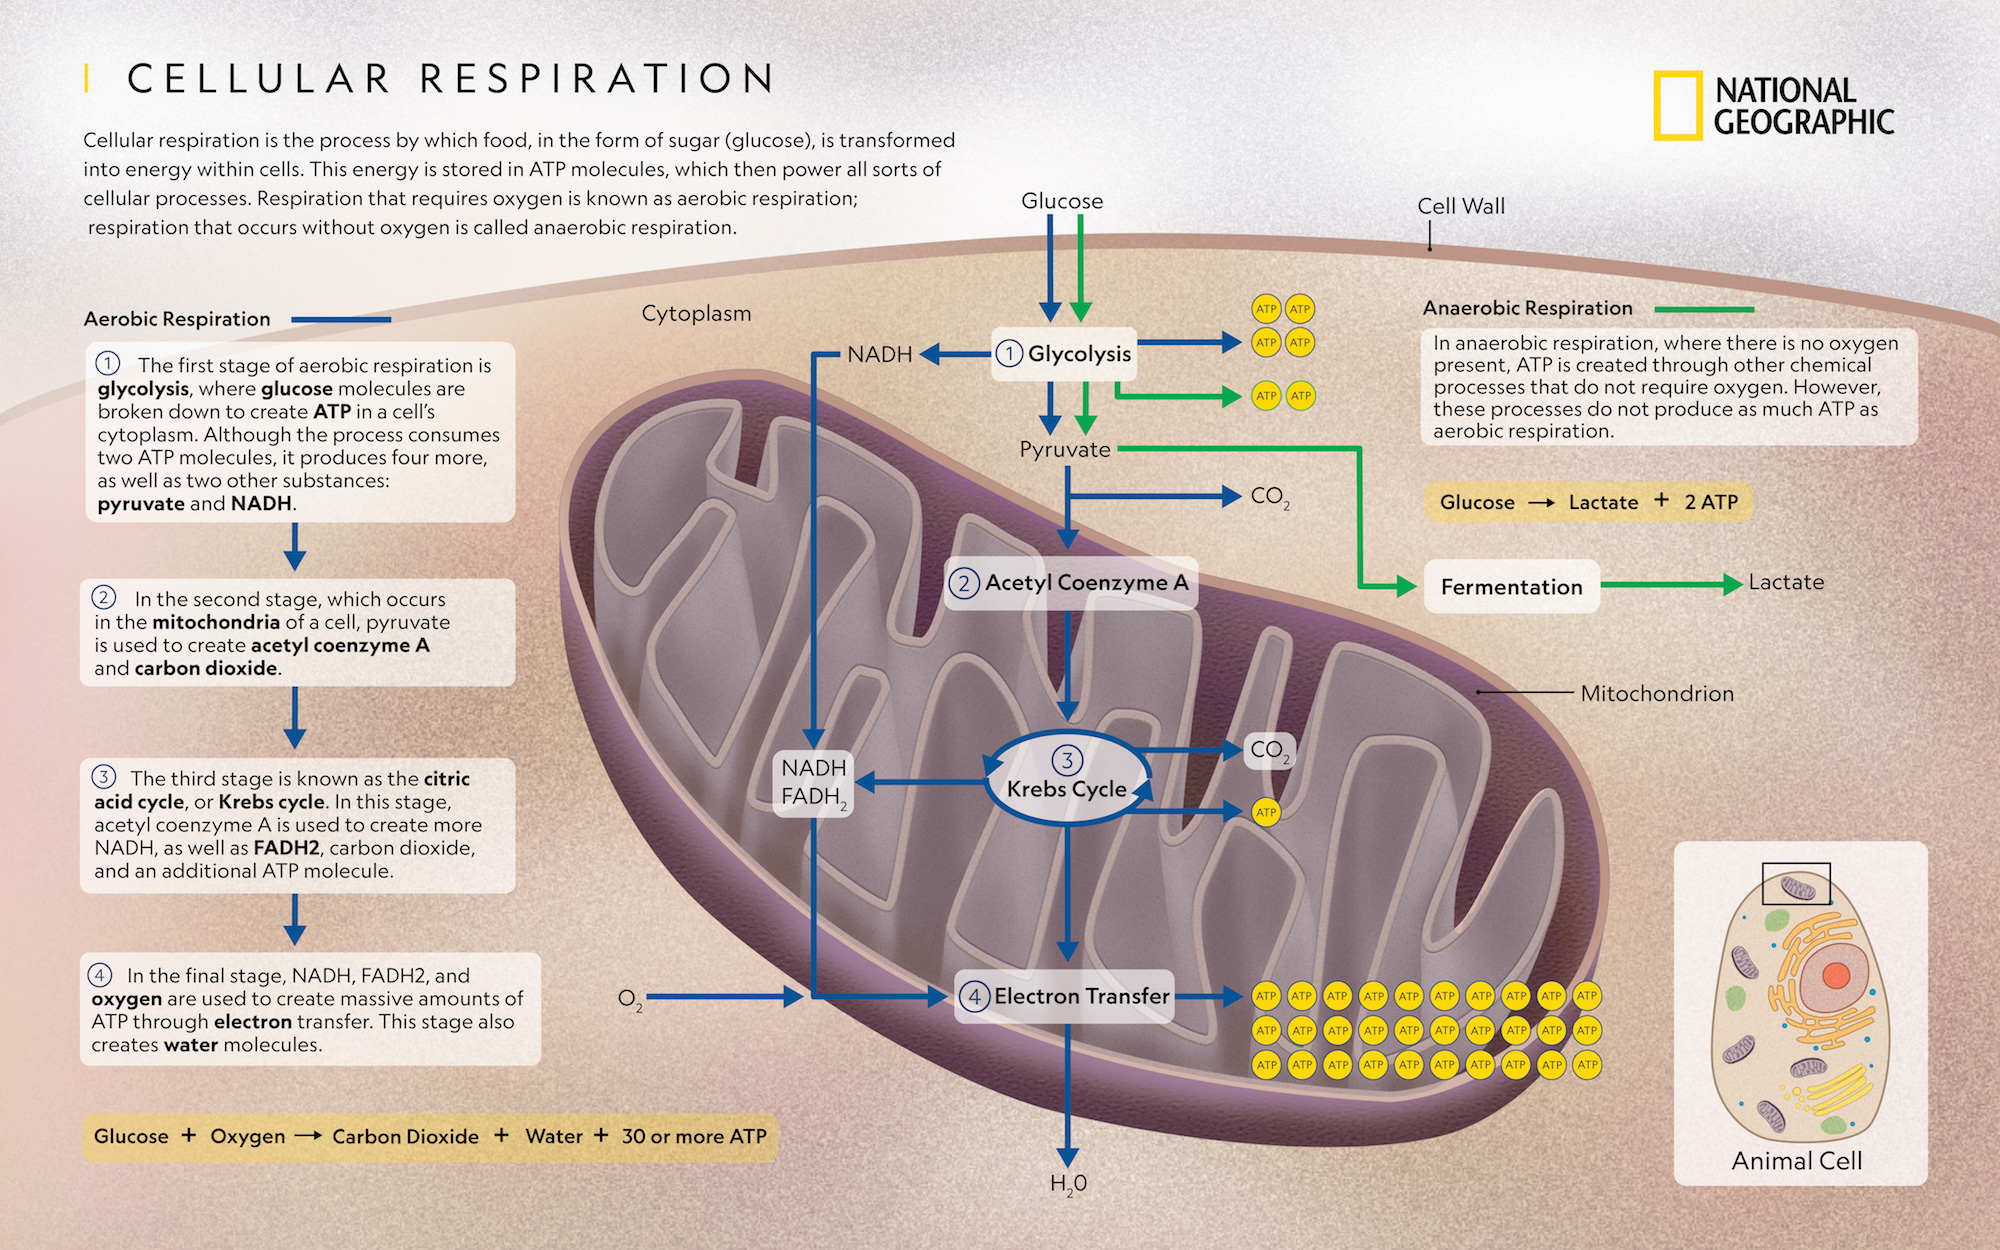
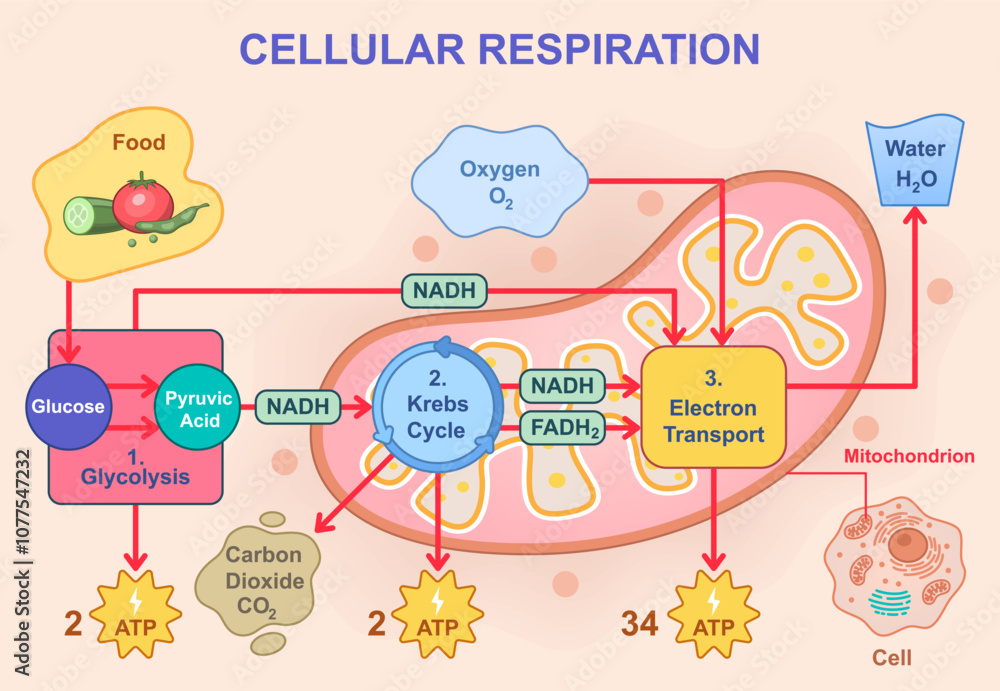
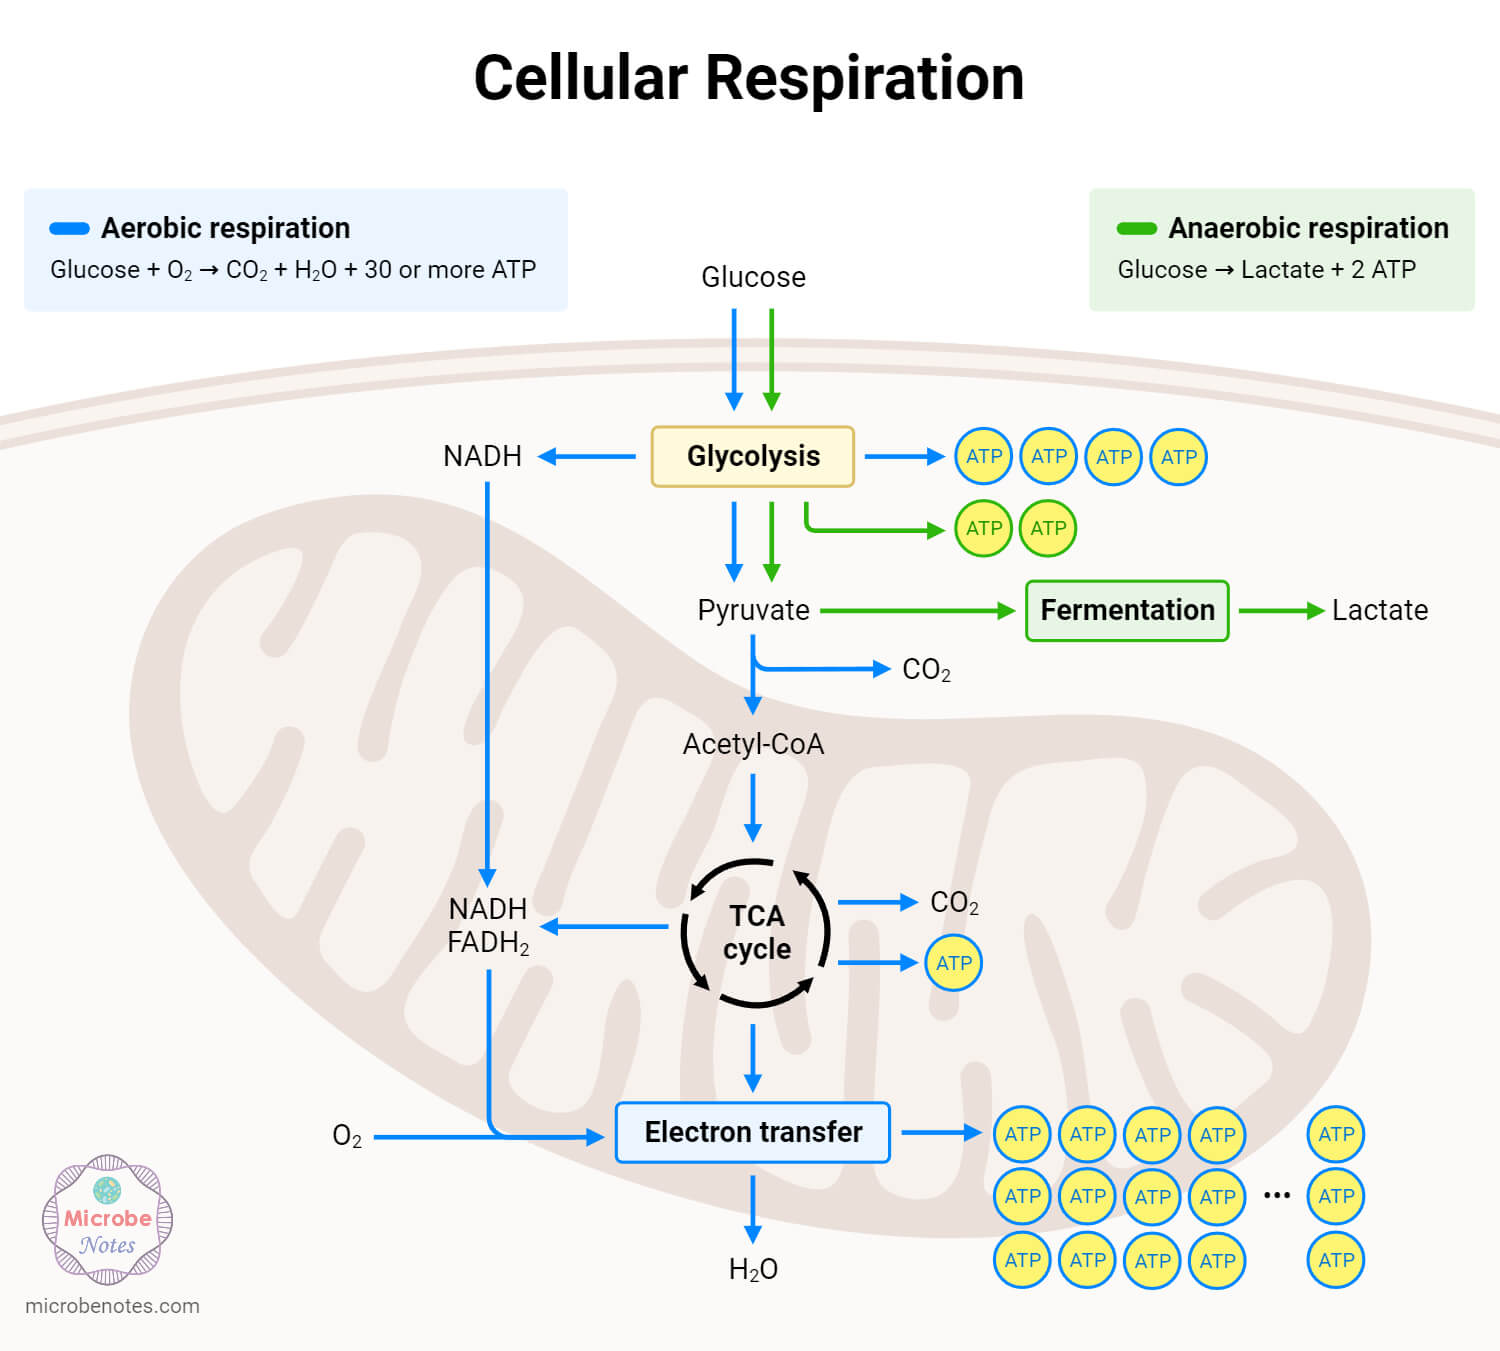
I spent three years teaching introductory biochemistry to undergraduates who couldn't tell the difference between glycolysis and the Krebs cycle. The most common question I got was whether cellular respiration happens in the cytoplasm or somewhere else. It turns out people have strong opinions about this, and most of them are wrong. The mitochondrion carries out the bulk of cellular respiration. Specifically, it handles the citric acid cycle, the electron transport chain, and oxidative phosphorylation. Glycolysis happens in the cytoplasm, but that only produces a net two ATP per glucose molecule. The mitochondrion generates roughly thirty more. That is the difference between keeping a cell alive and watching it slowly run out of energy. Here is what most textbooks leave out. The mitochondrion is not a standalone organelle doing its own thing. It exists in constant dialogue with the rest of the cell. Calcium signals from the endoplasmic reticulum modulate mitochondrial dehydrogenases. Reactive oxygen species produced during electron transport act as signaling molecules that trigger adaptive responses elsewhere. The organelle is embedded in a network of metabolic fluxes that no single diagram captures accurately.
The Mechanics of It
Glucose enters the cell and gets broken down through glycolysis into two pyruvate molecules. This occurs in the cytosol and produces a minimal amount of ATP through substrate-level phosphorylation. The pyruvate then crosses the inner mitochondrial membrane through the pyruvate carrier protein. Once inside, pyruvate dehydrogenase converts it to acetyl-CoA, which feeds into the citric acid cycle. The citric acid cycle runs eight enzyme-catalyzed reactions in the mitochondrial matrix. Each turn produces three NADH, one FADH2, one GTP, and releases two CO2 molecules. The NADH and FADH2 carry high-energy electrons to the electron transport chain embedded in the inner mitochondrial membrane. Complexes one through four pass electrons through a series of redox reactions, pumping protons from the matrix into the intermembrane space. This creates an electrochemical gradient across the inner membrane. ATP synthase, also known as complex five, uses the flow of protons back into the matrix to phosphorylate ADP into ATP. This process generates the majority of cellular ATP. A single glucose molecule yields approximately thirty to thirty-two ATP through oxidative phosphorylation, depending on the shuttle system used to transport cytoplasmic NADH into the mitochondrion.
What Beginners Miss
The first thing students get wrong is assuming the mitochondrion is the only site of ATP production. Glycolysis produces ATP without oxygen. Some cells, like red blood cells, lack mitochondria entirely and rely solely on anaerobic glycolysis. Cancer cells often prefer glycolysis even in the presence of oxygen, a phenomenon called the Warburg effect. They do this because glycolysis provides biosynthetic intermediates faster than oxidative phosphorylation, even though it is less efficient per glucose molecule. The second misconception is that mitochondria are identical across tissues. Brain mitochondria have different membrane compositions than liver mitochondria. Skeletal muscle mitochondria can switch between oxidative and glycolytic phenotypes depending on training status. Cardiac mitochondria occupy forty percent of cardiomyocyte volume and depend almost exclusively on fatty acid oxidation. These tissue-specific adaptations matter when you are trying to understand metabolic diseases.
Get the Full Details
A Problem I Encountered
I once worked with a researcher studying mitochondrial dysfunction in neuronal cells. We were measuring oxygen consumption rates using a Seahorse analyzer, and the data looked completely normal. The cells were respiring fine. But when we measured ATP levels, they were half of what we expected. The problem was that the cells were compensating through increased glycolysis. The mitochondria were functioning, but the overall energy output was insufficient. The workaround was to measure both parameters simultaneously and calculate the mitochondrial versus glycolytic ATP contribution. Only then did we see the full picture. This experience taught me that respiratory metrics alone are never sufficient. You need to understand the complete metabolic landscape before drawing conclusions about mitochondrial health.
Limitations and Where This Model Breaks
Oxidative phosphorylation is not a perfect system. The electron transport chain leaks approximately two percent of electrons to oxygen, producing superoxide radicals. These reactive oxygen species damage mitochondrial DNA, which lacks histone protection and has limited repair mechanisms. This damage accumulates with age and contributes to cellular senescence. The system also depends on a steady supply of ADP and inorganic phosphate. When ATP demand drops, the proton gradient increases and eventually becomes so large that electron transport cannot proceed efficiently. This is called respiratory control, and it prevents wasteful respiration when energy is not needed. But it also means that mitochondrial ATP production is tightly coupled to cellular energy demand. There is no buffer. Another limitation is the dependency on oxygen. Without it, the electron transport chain stops, the proton gradient collapses, and ATP synthase runs in reverse, hydrolyzing ATP instead of producing it. Cells survive this condition for a short time through anaerobic glycolysis, but most tissues cannot maintain function for more than a few minutes without oxidative phosphorylation.
Practical Implications
If you are studying cellular metabolism, start with the basics but do not stop there. Learn the enzyme names, the intermediate compounds, and the stoichiometry. Then move to the regulatory mechanisms. Allosteric regulation of phosphofructokinase by ATP and citrate controls glycolytic flux. Isocitrate dehydrogenase regulation by ADP controls citric acid cycle rate. These checkpoints determine whether the cell prioritizes energy production or biosynthesis. When designing experiments, measure multiple parameters. Oxygen consumption rate tells you about electron transport chain activity. ATP production rate tells you about overall energy output. Reactive oxygen species measurement tells you about mitochondrial stress. Membrane potential measurement tells you about proton gradient integrity. No single metric gives you the complete picture. The mitochondrion is often called the powerhouse of the cell, but that description is too simplistic. It is a metabolic integration hub that responds to cellular energy status, calcium signaling, oxidative stress, and apoptotic cues. Understanding it requires more than memorizing the citric acid cycle. It requires seeing how mitochondrial function connects to everything else in the cell.