The Reactants Behind Cellular Respiration (And Why Most People Get Them Wrong)
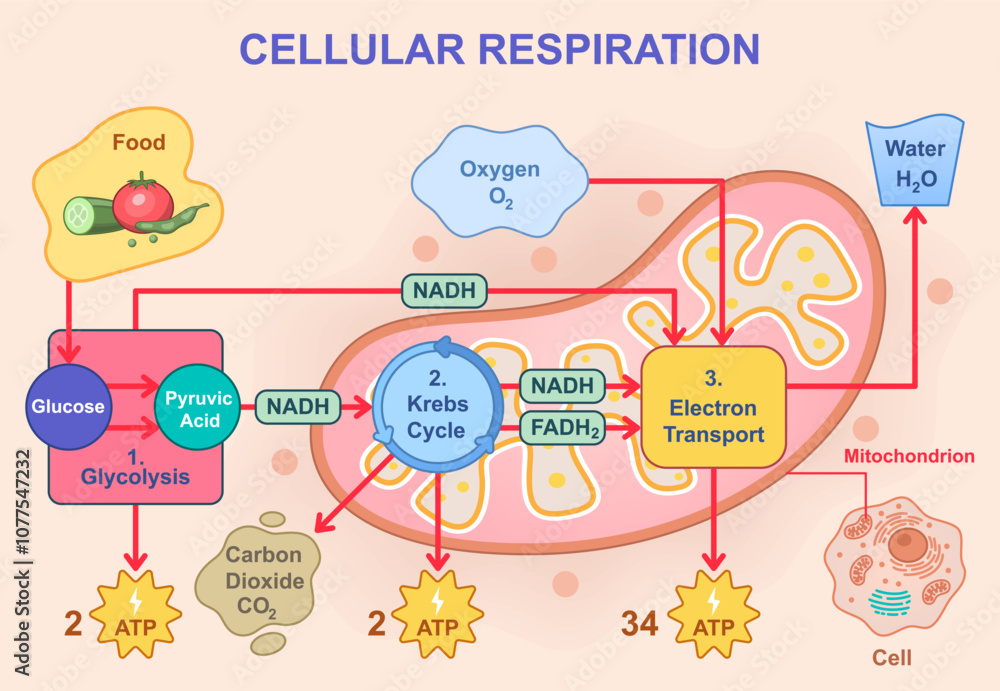
The balanced equation for aerobic cellular respiration is C6H12O6 + 6O2 6CO2 + 6H2O + ~30–32 ATP. That's glucose plus oxygen, yielding carbon dioxide, water, and usable energy. Most people stop there. The details matter more than the equation on a test. I used to teach this to introductory biology students, and there was one consistent failure point that drove me crazy. They'd memorize the equation perfectly and then struggle when asked what happens if oxygen drops below a certain threshold during glycolysis followed by the Krebs cycle. The answer isn't dramatic—it's that pyruvate gets shunted toward lactate fermentation instead of entering the mitochondria, and ATP yield collapses from roughly 30+ per glucose molecule down to just 2. I started making them trace individual carbons through the pathway instead of just reciting the overall reaction. It took about ten minutes longer per lab session, but their retention on the actual chemistry improved noticeably.
The Ultimate Fuel Source Uncovering The Reactants Of Cellular Respiration
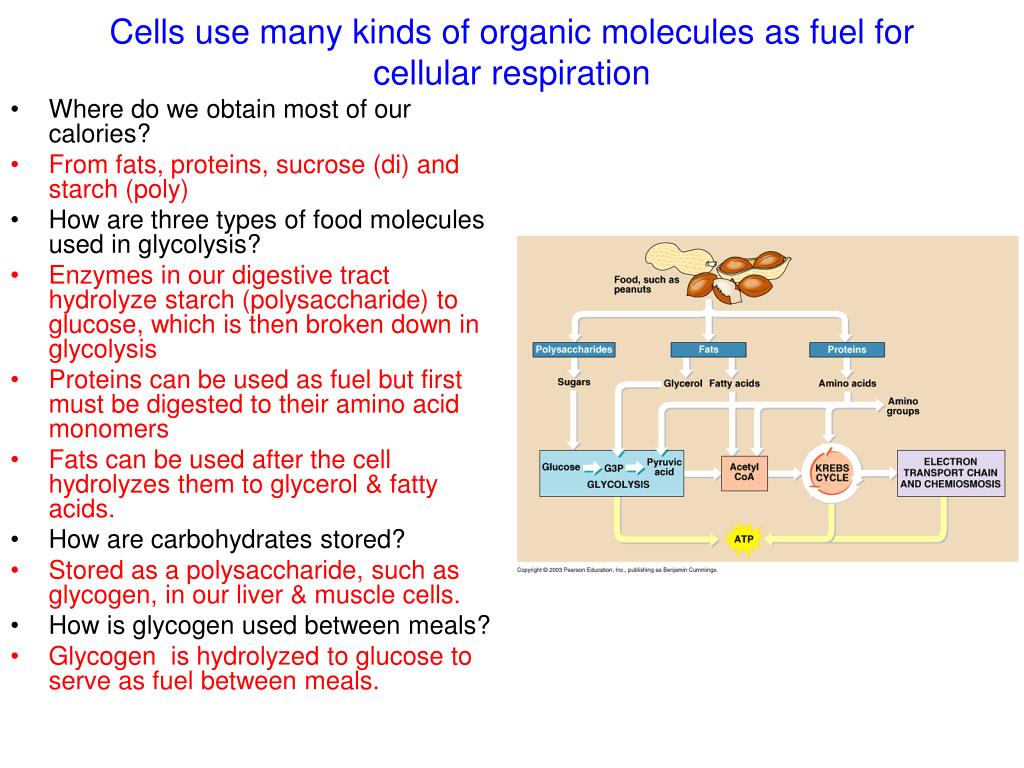
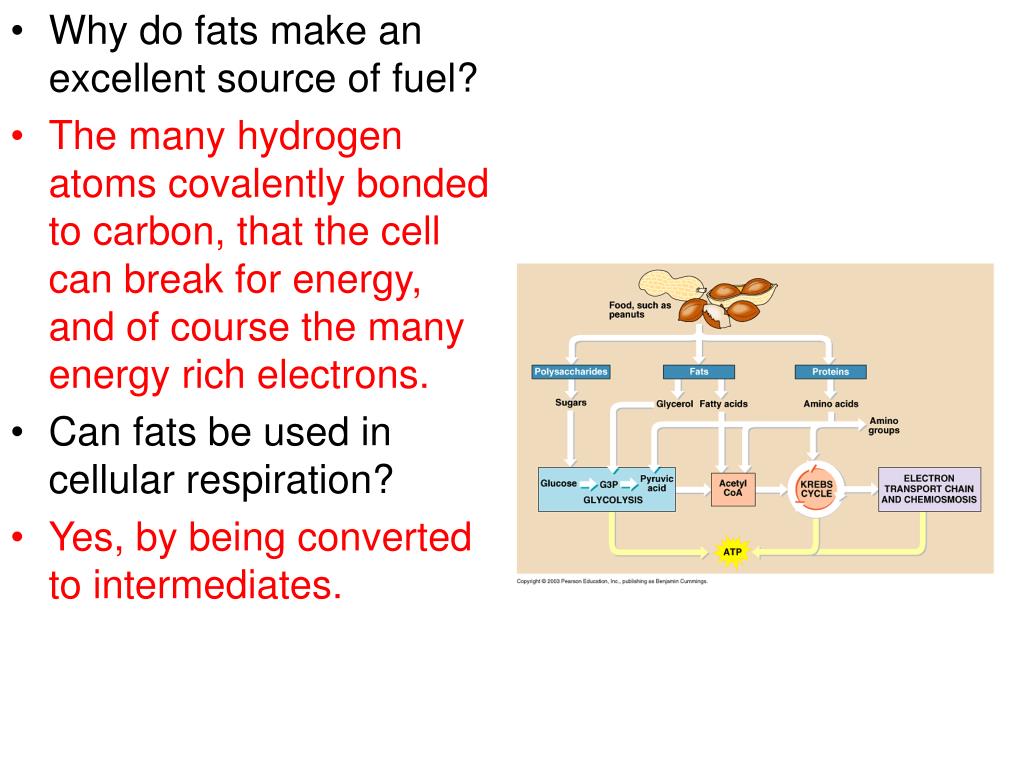
Glucose isn't the only fuel source, but it's the standard reference point. Fatty acids and amino acids can feed into the same pathway at various entry points. Acetyl-CoA derived from beta-oxidation enters right before the Krebs cycle. That's why long-chain fatty acids can produce more ATP per carbon than glucose does—more carbons to oxidize, more rounds of the cycle. Here's something most textbooks don't emphasize enough: oxygen isn't just some abstract "input" floating in the equation. It's the terminal electron acceptor at complex IV of the electron transport chain. Without it, the entire chain backs up. Protons can't be pumped across the inner mitochondrial membrane. The proton gradient dissipates. ATP synthase stops turning. That's why cyanide and carbon monoxide are lethal at the molecular level—they don't block glycolysis or the Krebs cycle directly; they sit at complex IV and paralyze the whole system. One edge case that comes up surprisingly often: people assume you measure glucose consumption and oxygen consumption at a 1:6 molar ratio in real experimental setups. In practice, it's never exactly 1:6 because cells often use alternative substrates simultaneously, and some glucose carbons get diverted into biosynthetic pathways like the pentose phosphate shunt instead of fully oxidized. When I ran respirometry labs, the measured respiratory quotient (CO2 produced divided by O2 consumed) for pure glucose oxidation should be 1.0. If your RQ came out as 0.85, you had lipid oxidation happening alongside. If it was 0.7, pretty much everything being burned was fat. That number alone tells you what the cell is actually fueling itself with at any given moment.
The practical constraint worth understanding is that this whole process is limited by mitochondrial density and membrane integrity. A sedentary person's muscle cells have roughly a third of the mitochondrial count of an endurance athlete's. More mitochondria means more surface area for the electron transport chain complexes, which means more proton gradient capacity, which means more ATP per unit of time. Training adaptations don't change the reactants—they change the infrastructure that processes them. There's also a common misconception about where water comes from in the equation. It's not a product of the Krebs cycle itself. It's formed when electrons from NADH and FADH2 reach oxygen at the end of the electron transport chain. The water produced this way actually contributes to the body's total water pool. Not a dramatic insight, but the source matters more than you'd guess when someone asks where cellular water comes from.
Get the Full Details
What You Actually Need to Track in Practice
If you're running any kind of experiment or trying to model this system, focus on four things: the amount and type of substrate available, oxygen concentration in the environment, mitochondrial health indicators, and the downstream demand for ATP. The reactants are simple. The regulation around them is what determines whether you're running efficiently or just burning fuel without getting much done. Starvation states flip the whole thing. Glucose runs out. The body shifts to ketone bodies and free fatty acids. The reactants change, the pathway adapts, but the core machinery—the same complexes, the same proton gradient, the same ATP synthase—keeps running. It's just feeding off a different tank. That's essentially it. The reactants are glucose and oxygen. Everything else is detail work.