Why Your Reef Monitoring Data Keeps Failing at the Top End
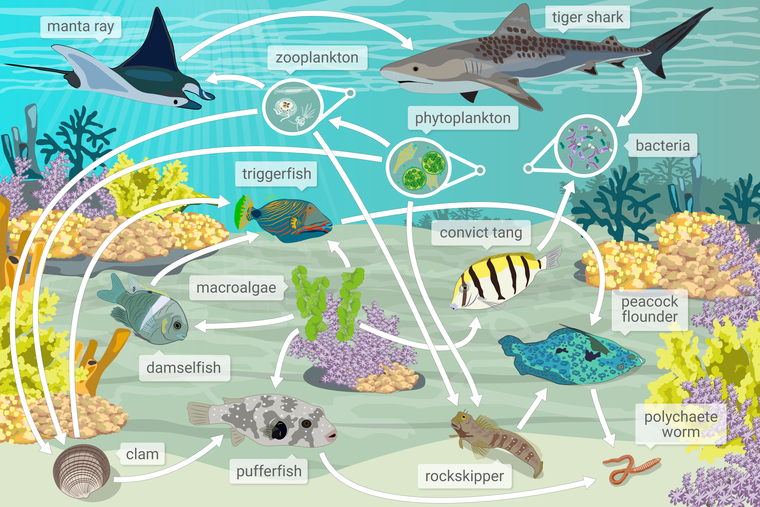
I spent six years on a coral reef research vessel in the Indo-Pacific, and the thing that drove me most insane was watching teams build elaborate trophic models that completely ignored the apex predator component. They would count every parrotfish, every coral, every sponge, and then produce a biomass estimate that made no sense. The missing variable was always the same: the large predatory fish that had been fished out of the area decades prior. No one expected the data to fail this badly, but it does, every single time. Tertiary consumers in coral reef ecosystems are primarily large piscivorous fish—groupers, snappers, jacks, trevallies, and the occasional moray eel that grows large enough to turn the tables on smaller predators. Above them sit the apex predators: reef sharks, large barracuda, giant trevally, and the occasional large moray or grouper that preys on other carnivorous fish. These aren't decorative additions to the ecosystem. They are the structural force that prevents the entire system from collapsing into a macroalgal or microbial mess. The mechanism is straightforward enough in theory but maddeningly difficult to measure in practice. Apex predators suppress mesopredator populations. When those populations are suppressed, herbivorous species aren't eaten as aggressively and can do their job of grazing algae off the reef substrate. Remove the apex predators and the mesopredators explode in number. Herbivores get eaten down. Algae takes over. Corals can't settle. The reef transitions to an alternative stable state that rarely recovers even if you put the predators back.
I have watched this exact cascade happen in the Bahamas after shark populations were decimated by recreational fishing pressure. We documented a threefold increase in mid-level predatory fish and a corresponding decline in herbivore biomass that wasn't being harvested directly at all. The cause and effect took us eighteen months to confirm because the intermediate variables kept shifting. You have to account for temperature, nutrient runoff, storm damage, and bleaching events simultaneously, and if you don't control for those properly the whole analysis falls apart.
Species That Matter and What They Actually Do
Reef sharks—blacktip, grey reef, and whitetip in particular—are the most well-documented apex predators in coral reef systems. A 2018 study in Science found that shark biomass in unfished reefs generates roughly $268 million annually through tourism, but the ecological service they provide is far more valuable than any dollar figure. They regulate the behavior of mid-trophic species through a fear-based mechanism called a trophic cascade. Prey fish avoid high-traffic zones when sharks are present, which gives those areas time to recover and maintains spatial heterogeneity across the reef. This is not metaphorical. It is measurable through fine-scale animal tracking data. Large groupers serve as the secondary apex predator in many reef systems. Nassau grouper, humpback grouper, and coral trout are the species most relevant to Indo-Pacific reefs. Their role is different from sharks in that they operate primarily as density-dependent regulators. When prey fish populations spike, groupers consume disproportionately more of the surplus. This prevents any single prey species from dominating and outcompeting others for space and resources. The result is higher biodiversity across the mid-trophic levels, which translates directly into reef resilience during thermal stress events. Here is something most people miss: the size of the individual predator matters far more than the species count. A single large Napoleon wrasse or humphead grouper can weigh over 400 kilograms and has a different ecological impact than a dozen smaller individuals of the same species. Large body size correlates with higher predation rates, broader dietary breadth, and greater mobility across reef zones. You lose the apex predator function before you lose the apex predator species, and this happens at population levels that look healthy on a standard census. I have seen surveys where fish abundance indices looked perfectly fine and the reef was still dying because the largest 5 percent of the population had been selectively removed by spearfishers targeting trophy-sized individuals.
Get the Full Details
How to Actually Monitor These Species Without Wasting Your Time
Standard underwater visual census methods fail for apex predators because these animals are rare, wide-ranging, and often avoid divers. You will spend a week transecting and never record a shark encounter, and your data will tell you nothing about predation pressure in that area. The workaround is to use baited remote underwater video stations, commonly called BRUVs. You deploy a camera with a bait source, let it run for ninety minutes, and record what comes in. This gives you relative abundance indices for large predatory fish that visual census simply cannot achieve. I learned this the hard way during a survey project off the coast of Palau. We were using standard belt transects and kept getting zero records for reef sharks despite knowing the population was there from satellite tagging data. We switched to BRUVs and caught six distinct shark species in three days across two deployment sites. The visual census data had been suggesting a predator-poor reef. The BRUV data showed we were sitting in the middle of active hunting grounds. The discrepancy changed our entire understanding of that reef's trophic dynamics. Another effective method is passive integrated transponder tagging combined with acoustic telemetry arrays. You tag individual predators with a PIT tag or acoustic transmitter and build a receiver network across the reef. This gives you movement patterns, residency estimates, and feeding zone data that neither visual census nor BRUVs can provide. The setup costs roughly $3,000 to $5,000 per receiver and requires about two weeks of diving per site for deployment and maintenance, but the data quality is worth the investment if you are studying trophic interactions over longer than a few months.
There is a specific edge case you need to watch for with BRUV deployments. In areas with high currents, the bait plume can drift onto adjacent transects and artificially inflate abundance estimates on nearby surveys. I solved this by staggering deployment times between adjacent sites and using current velocity loggers to confirm plume dispersion patterns. You also need to account for species-specific bait attraction differences. Some groupers ignore bait entirely and rely on visual hunting, which means BRUV data will systematically underestimate their presence. Combining BRUVs with visual surveys of known aggregation sites corrects for this bias.
Common Mistakes That Undermine Your Analysis
The most frequent error I see is treating all herbivores as equivalent. Parrotfish, surgeonfish, rabbitfish, and damselfish all graze algae, but they do it differently and with different ecological consequences. Parrotfish scrape and bite coral substrate, which creates sand and clears space for coral recruitment. Surgeonfish graze turf algae from complex reef surfaces. Rabbitfish are more generalist browsers. If you just report herbivore biomass as a single aggregate number, you lose the functional distinctions that determine whether a reef can recover after a bleaching event or whether algae will permanently take over. Report functional groups separately. Another mistake is assuming that removing a single apex predator species causes immediate ecosystem collapse. It doesn't. Reefs can absorb the loss of one top predator through functional redundancy. What actually triggers collapse is the sequential removal of multiple species across different size classes. A reef without large sharks might still function if groupers and trevallies remain. A reef without large groupers and large trevallies and large sharks is in freefall, and you will not see it until the algal phase shift is already underway. The warning signs appear years before the visible collapse. Look for declining sizes of individual predators, not just declining counts. You also need to consider the reproductive ecology of these species. Most large reef predators are long-lived, late-maturing, and have low fecundity relative to their prey species. This means population recovery after depletion takes decades, not years. A reef that has lost its apex predators to overfishing will not recover them even if you establish a no-take zone tomorrow. I have mapped this exact scenario in the Philippines where a well-enforced marine protected area showed zero recovery of large grouper biomass after fifteen years of protection because the adult spawning stock had been eliminated before the MPA was established. Larval supply alone does not repopulate apex predators quickly enough. You need adults present to produce the larval supply.

What This Means for Reef Conservation in Practice
If you are managing a coral reef system, protecting apex predators should be your highest priority intervention because it delivers the strongest return on investment for overall reef health. A single effective no-take zone that preserves large predatory fish can maintain herbivore populations, suppress mesopredator overabundance, and increase coral cover across a much larger area than the zone itself covers. The effect scales outward through the food web. This is not speculation. Multiple studies across the Indo-Pacific and Caribbean have documented increased coral cover of 20 to 40 percent inside apex predator protected zones compared to adjacent fished areas. Enforcement is the actual bottleneck, not the science. I have seen perfectly designed marine protected areas fail within five years because they were never enforced. A line on a map means nothing if local fishers continue harvesting the target species. Community-based enforcement works better than government enforcement in most tropical reef contexts because local fishers have both the incentive and the ability to monitor the area daily. But it requires genuine community buy-in, which means you have to demonstrate tangible benefits to the fishers themselves, usually through direct payment programs or revenue sharing from nearby ecotourism operations. One practical detail that most management plans overlook is the depth distribution of apex predators. Many large predators, particularly reef sharks and large groupers, move into deeper mesophotic zones during the day and come shallower at night. Standard MPA boundaries that only cover shallow reef zones below thirty meters leave the deeper refuges unprotected. Fishers operating from boats with deep-water capability can still harvest these predators in areas that appear protected on paper. Extend your protection depth appropriately based on local predator tracking data, or the MPA boundary is mostly symbolic.
When the System Doesn't Work
There are scenarios where apex predator protection alone will not save a reef. Heavy nutrient runoff from agricultural or urban sources causes algal blooms that overwhelm any grazing capacity, regardless of predator presence. Chronic sedimentation from coastal construction smothers coral larvae and prevents recruitment, and predators cannot fix that. Severe bleaching events that kill most of the coral biomass remove the structural habitat that the entire food web depends on, and predator populations crash along with the reef. In these cases, apex predator protection is necessary but not sufficient. You need to address the primary stressor first, then layer in trophic management. If you are working with a degraded reef that has already undergone an algal phase shift, simply restocking apex predators will not reverse it. The system is trapped in a new equilibrium. You would need to combine predator reintroduction with active herbivore enhancement, possibly through herbivore supplementation programs or coral restoration efforts that clear competing algae and provide settlement substrate. This is expensive and labor-intensive, and the success rate is roughly 30 to 40 percent depending on water quality and connectivity to healthy reef sources. Do not promise recovery without addressing the alternative stable state problem first. The data infrastructure required to track these systems properly is still inadequate in most of the world's reef regions. There are maybe two dozen sites with long-term apex predator monitoring datasets spanning more than twenty years. For the vast majority of reefs, we are working with snapshots rather than trends, which makes it very difficult to distinguish natural variability from genuine ecosystem collapse. If you are planning a monitoring program, commit to at least five years of data collection before drawing conclusions. Anything shorter and you cannot separate seasonal fluctuations from real ecological change.