What Actually Happens Inside Fatty Acid Synthase
When you first look at a biochemistry paper on fatty acid synthase, it reads like a factory assembly line. You start with acetyl-CoA and malonyl-CoA, you add two carbon units at a time, and you end up with palmitate. That's the textbook version. The real enzyme is a bit messier than that. I spent a semester working with recombinant FAS from Escherichia coli and E. coli FAS is a type I fatty acid synthase, meaning the whole complex is essentially one large polypeptide chain with multiple catalytic domains fused together. Not like type II systems where each enzyme is separate, as in bacteria and plants. The fused architecture matters because it changes how substrate channels work, how you purify the thing, and why your activity assays sometimes look wrong.
The Secret To Life Unraveling The Mysterious Fatty Acid Synthase Enzyme
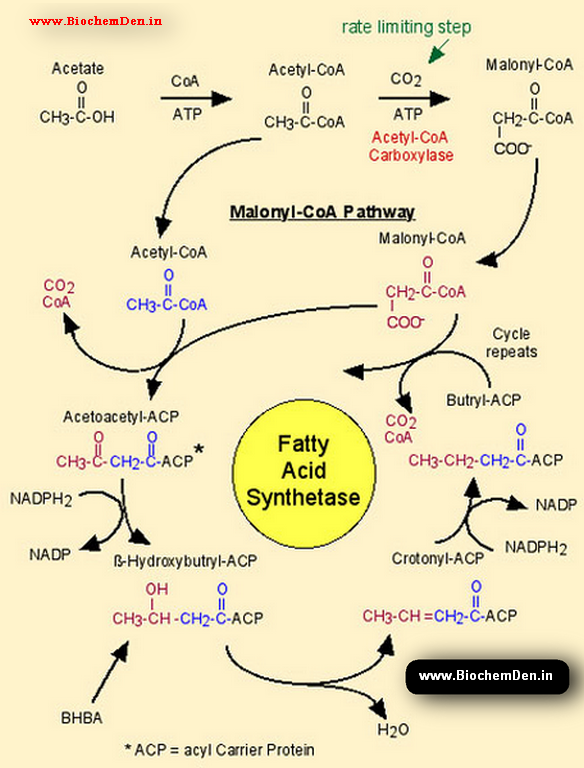
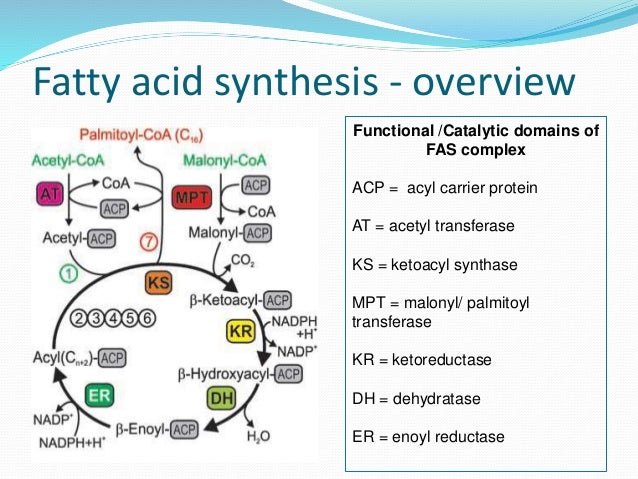
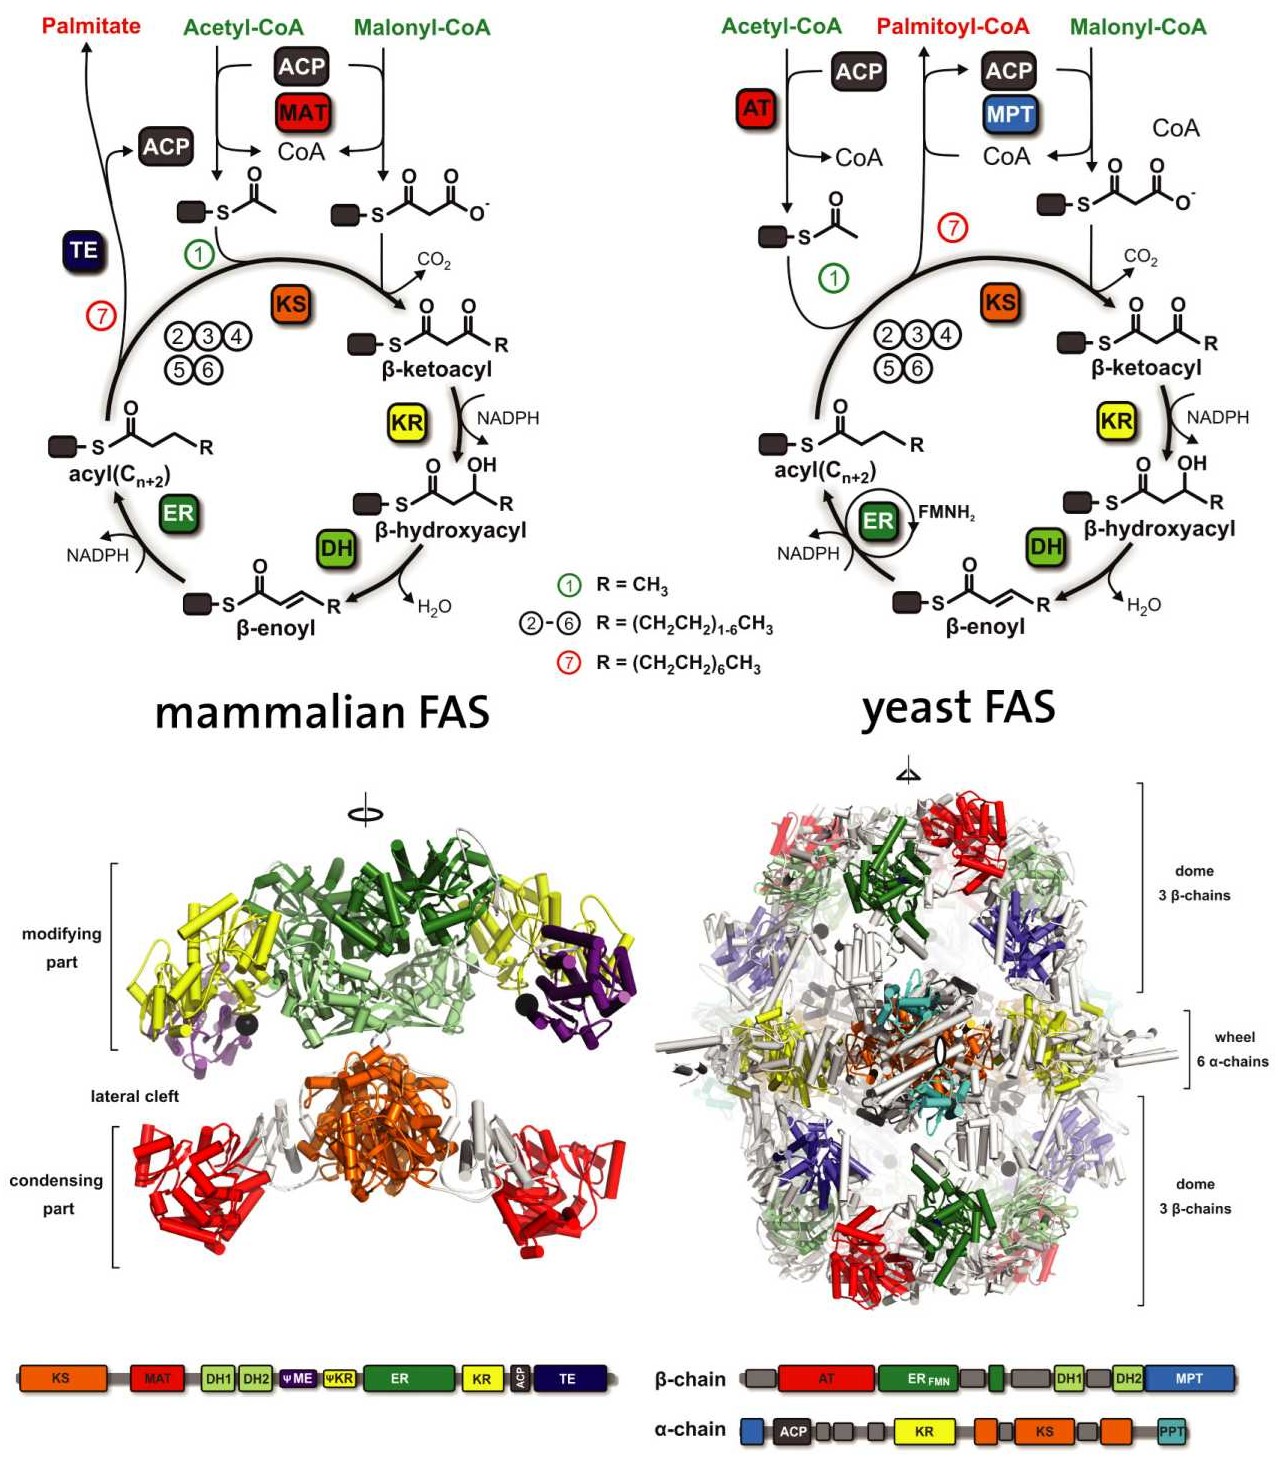
That phrase sounds like something out of a popular science magazine, but stripped of the marketing language it points at something real. Fatty acid synthase is central to how cells build lipids, and understanding its mechanism has implications from antibiotic development to metabolic disease research. The enzyme sits at the crossroads of energy storage and membrane biosynthesis. When it dysregulates, you get problems like the lipotoxicity seen in certain forms of diabetes or the altered membrane composition in some cancers. Here's the part most summaries skip over. The iterative elongation cycle runs through four chemical steps repeated over and over. First you have condensation where the ketosynthase domain joins an acyl group to a malonyl group releasing CO2. Then reduction by the ketoreductase domain turning that beta-keto group into a beta-hydroxyl. Then dehydration by the dehydratase removing water to form an enoyl intermediate. Then a second reduction by the enoyl reductase using NADPH to saturate the bond. Each round adds two carbons. The carrier protein in the middle is the acyl carrier protein or ACP and it shuttles the growing chain between domains via a phosphopantetheine arm. That prosthetic group gets loaded during maturation by a separate enzyme called a phosphopantetheinyl transferase. If your recombinant protein isn't getting post-translationally modified properly, your FAS will express fine but show almost no activity in assays. That was my first week of headaches.
Structure Matters More Than You'd Expect
Type I FAS in mammals forms a huge dimer of two large chains. Each chain carries all the catalytic activities. The structure looks roughly spherical under electron microscopy, about 250 kilodaltons per monomer giving a 500 kilodalton holoenzyme. The catalytic domains arrange themselves so the ACP can swing between active sites without the substrate ever leaving the complex. This channeling effect is why the enzyme is so much more efficient than mixing individual pure enzymes in a tube. In bacteria like E. coli, the system is completely different. Type II FAS uses discrete monofunctional enzymes. FabB FabF for condensation FabZ or FabA for dehydration and so on. That distinction isn't just academic because it affects how you'd approach inhibiting the enzyme. Broad-spectrum antibacterial strategies targeting type II FAS have been explored but hitting the right Fab enzyme without affecting human metabolism turned out to be trickier than the initial papers suggested.
Get the Full Details

Purification And Activity Assays: Where Things Go Wrong
If you're actually working with this enzyme and not just reading about it, here's a practical note. Commercial FAS preparations or your own overexpressed protein can lose activity fast if you're not careful about the phosphopantetheinylation step. Native FAS gets modified in the cell. Recombinant FAS expressed in standard BL21(DE3) cells often comes out apoprotein, meaning the ACP domain lacks that essential arm. You need to supplement with a phosphopantetheinyl transferase like Sfp during purification or do an in vitro labeling step with coenzyme A and the transferase after you've isolated the protein. Activity assays typically measure NADPH consumption at 340 nanometers or use radiolabeled acetyl-CoA and track product formation by thin layer chromatography. The spectrophotometric method is faster but it has a blind spot. NADPH is consumed in two of the four steps, not just one, so the stoichiometry isn't straightforward. You have to account for the fact that each full cycle turns over two NADPH molecules per two carbons added. If you're comparing wild type to a mutant, make sure you're normalizing to active holoenzyme not just total protein by Bradford or BCA, because those don't tell you whether your ACP is actually modified.
Common Misunderstandings About FAS Regulation
One thing I see people get wrong is assuming FAS activity maps directly to citrate levels. Citrate allosterically activates acetyl-CoA carboxylase which makes malonyl-CoA, the substrate donor for FAS. So citrate indirectly feeds the system. But FAS itself isn't primarily regulated by allosteric effectors in most tissues. The real control points are transcriptional, through sterol regulatory element binding proteins and insulin signaling pathways, and through substrate availability. Post-translational regulation is more about the phosphorylation state of upstream ACC than about FAS itself. Another trap is thinking that because FAS makes palmitate the product it's done. Palmitate then gets elongated by elongases in the endoplasmic reticulum or desaturated by desaturases to make oleate and other longer chains. FAS is the starter, not the finish line. If your question is about membrane lipid composition or signaling molecules like palmitoylated proteins, you need to think beyond the synthase complex itself.
Inhibitors And Therapeutic Angles
Orienteerin and its analogs were discovered as natural products that target the ketosynthase domain. They covalently modify a catalytic cysteine residue and shut down condensation. That sounds clean but in practice the selectivity between microbial and mammalian FAS is moderate because the active site architecture shares conserved features. The bigger therapeutic interest has shifted toward cancer metabolism, where FAS is often overexpressed in tumor cells and supports rapid membrane biogenesis. Small molecule inhibitors like TVB-2640 moved into clinical trials for solid tumors. The limitation nobody likes to advertise is that systemic FAS inhibition causes metabolic side effects. Mammalian cells can compensate partially by oxidizing fatty acids instead of making them, but chronic suppression hits liver and muscle lipid handling. If you're designing an experiment around FAS inhibition, plan for compensatory metabolic rewiring and measure both de novo lipogenesis and fatty acid oxidation to get the full picture.

What I Wish I'd Known Earlier
The biggest practical lesson is that FAS is finicky outside of its native membrane environment. It's a multi-domain enzyme with hydrophobic regions and a mobile arm that depends on proper folding. Detergent choice matters more than you'd guess. Mild non-ionic detergents like NP-40 or digitonin tend to preserve activity better than stronger ones. Salt concentration, glycerol content, and avoiding repeated freeze-thaw cycles all influence how long your prep stays functional. I stopped trying to push specific activity numbers past two weeks and just learned to work fresh or store aliquots at minus eighty with 10 percent glycerol. The enzyme is a legitimate target and a legitimate model system for studying multi-domain catalysis. It doesn't need mystique attached to it. You just need to respect the biochemistry and the post-translational modifications or you'll spend weeks wondering why your absorbance trace is flat.