Why Glucose Matters More Than You Probably Realize
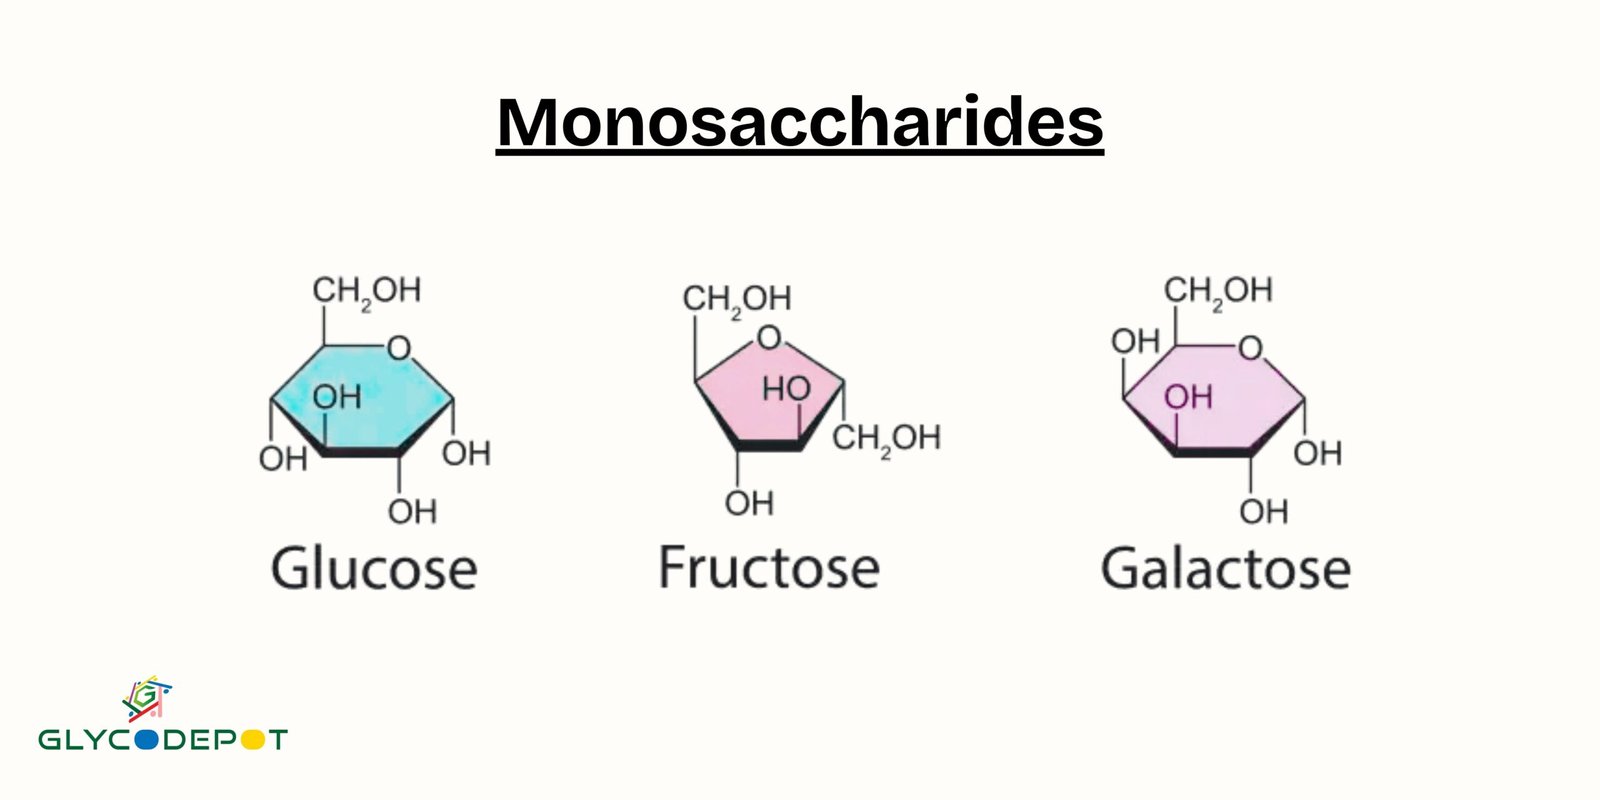
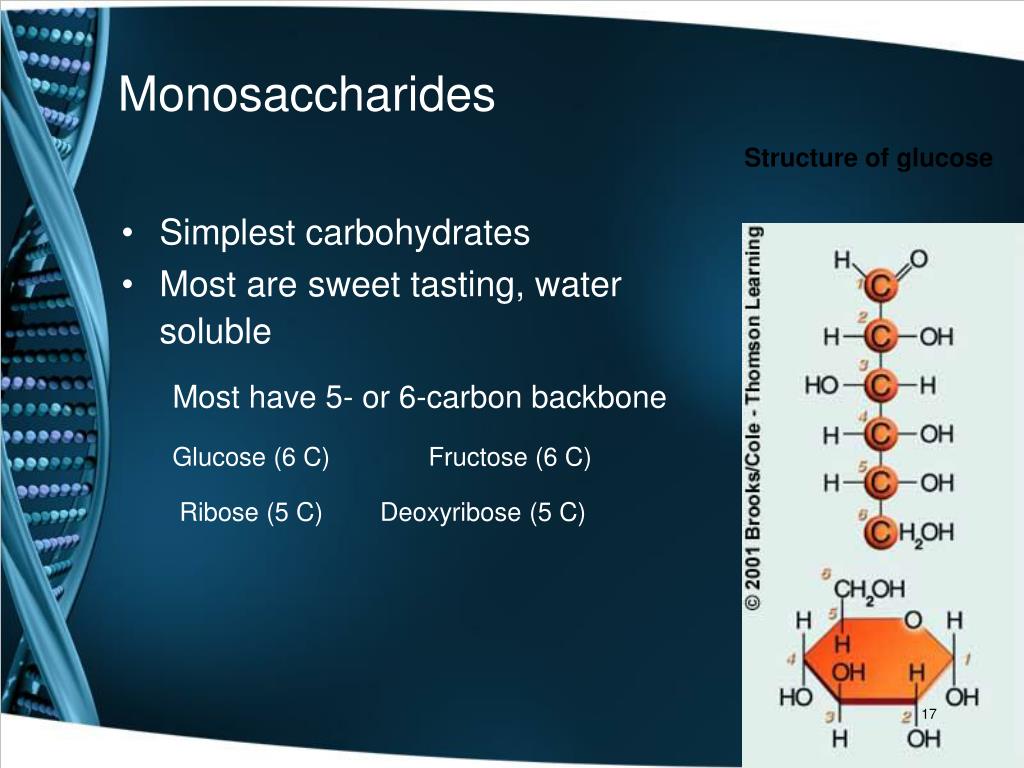
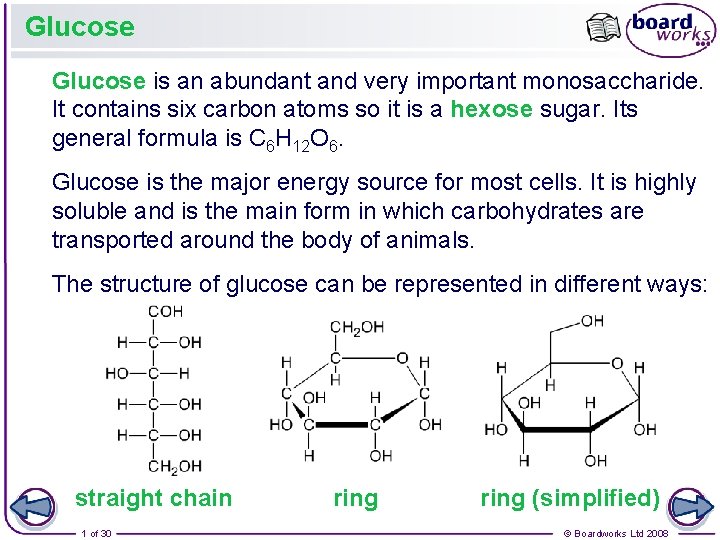
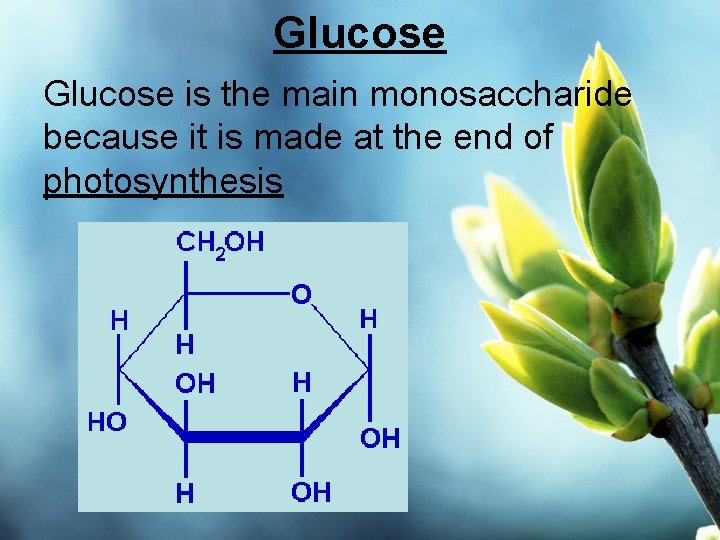
Glucose is the most abundant simple sugar in biological systems. It shows up everywhere from blood plasma to plant cell walls, and understanding it properly matters more for biochemistry, nutrition, and even industrial chemistry than most people give it credit for. I spent years working with carbohydrate analysis in a lab setting, and the thing that consistently trips people up is not the basic definition—it is the structural behavior of glucose in solution and how that affects everything from blood testing to fermentation outcomes. At the molecular level, glucose has the formula C6H12O6. That part is standard textbook material. What actually matters in practice is that glucose exists primarily as a ring structure in aqueous solution, not as the straight-chain form you see drawn in introductory diagrams. About 99% of glucose molecules in water adopt either the alpha or beta pyranose ring form, and they constantly interconvert through a process called mutarotation. The straight-chain aldehyde form is essentially a transient intermediate. This detail is critical because it determines how glucose reacts with enzymes, how it binds to proteins, and how analytical methods detect it. The ring closure creates a new stereocenter at carbon 1, which is why alpha and beta anomers exist. Alpha glucose has the hydroxyl group on carbon 1 pointing down relative to the ring plane, while beta glucose has it pointing up. Enzymes are picky about which anomer they process. Beta-glucosidases only handle the beta form. Alpha-amylase targets alpha linkages in starch. If you ignore this distinction in a practical setting, your reaction yields will be inconsistent and you will waste reagents chasing down problems that have nothing to do with concentration and everything to do with anomeric specificity.
I ran into this directly when troubleshooting a fermentation protocol for a biotech project. We were seeing inconsistent ethanol yields across batches, and the glucose concentration readings from our spectrophotometer kept varying by 8 to 12 percent even though we were adding the same nominal amount each time. The issue turned out to be that we were using D-glucose from a batch that had been stored improperly, allowing partial caramelization and anomer shift over time. The old stock had accumulated significant amounts of hydroxymethylfurfural from thermal degradation. Switching to freshly opened reagent-grade glucose and running a quick HPLC check before each batch resolved the inconsistency completely. You would think storing sugar in a cabinet would be fine, but carbohydrates degrade in ways that are not obvious without analytical confirmation.
How Glucose Functions in Biological Systems
In animals, glucose circulates in the blood at a tightly regulated concentration, typically between 70 and 100 milligrams per deciliter in fasting humans. The body uses insulin and glucagon to maintain this range. Cells take up glucose through transporter proteins, with GLUT4 being the insulin-responsive version found in muscle and fat tissue. Inside the cell, glucose enters glycolysis, producing pyruvate and generating ATP through oxidative phosphorylation. A single glucose molecule can yield approximately 30 to 32 ATP molecules under aerobic conditions, though this number varies depending on the shuttle system used to transport electrons into the mitochondria. Beyond energy production, glucose serves as a structural precursor. It is the monomer unit in glycogen for short-term storage in animals and in cellulose and starch for energy storage in plants. The difference between these polymers comes down to the glycosidic bond type. Starch uses alpha-1,4 linkages that humans can digest. Cellulose uses beta-1,4 linkages that require specialized enzymes most animals, including humans, do not produce. This single bond difference explains why cellulose passes through the digestive tract as fiber while starch becomes glucose. Glycosylation is another major function that people overlook. Glucose and its derivatives are attached to proteins and lipids on cell surfaces, forming glycoproteins and glycolipids that are essential for cell recognition, immune response, and signaling. Aberrant glycosylation patterns are associated with cancer metastasis and several genetic disorders. When you are studying glucose in a research context, keeping glycosylation in mind prevents you from treating it as nothing more than a fuel molecule.
Get the Full Details
Pitfalls and Limitations in Practical Applications
One of the most common mistakes I see in laboratory and clinical settings is assuming that all glucose measurement methods are interchangeable. Colorimetric assays based on the gluc oxidase reaction are convenient and inexpensive, but they can be interfered with by substances like acetaminophen, uric acid, and ascorbic acid at high concentrations. If you are working with blood samples from patients on certain medications, a colorimetric reading might look perfectly normal while the actual glucose level is significantly different. I encountered this when a clinic switched to a cheaper assay kit and started reporting deceptively normal glucose values for patients on high-dose vitamin C therapy. The ascorbate was interfering with the peroxidase step of the reaction. Switching to an enzymatic method with better specificity corrected the problem, but it took several weeks of retrospective chart review to catch it. Another limitation is that glucose stability in solution is not guaranteed. In buffered aqueous solutions, glucose undergoes slow degradation through Maillard reactions if amino acids are present, and through oxidation if the solution is exposed to air over extended periods. For long-term storage of glucose standards, you should aliquot and freeze the solutions rather than keeping them at room temperature. Even then, repeated freeze-thaw cycles promote degradation. I used to prepare weekly stocks and assumed they were stable, which led to subtle drifts in calibration curves that I attributed to instrument variability. Once I started making fresh monthly stocks and storing them at minus twenty degrees Celsius in single-use aliquots, the calibration stability improved noticeably. There is also the issue of optical rotation measurements. Glucose is dextrorotatory, which is why it is sometimes called dextrose. The specific rotation changes during mutarotation as the alpha and beta anomers equilibrate. If you are using polarimetry to measure glucose concentration, you need to allow the solution to reach equilibrium before taking a reading, or you need to control the timing precisely. Skipping this step introduces error that is difficult to diagnose because it looks random rather than systematic.
Industrial and Nutritional Considerations
On an industrial scale, glucose is produced primarily through the hydrolysis of starch from corn, wheat, or cassava. The process involves treating the starch with acids or enzymes to break the alpha-1,4 and alpha-1,6 glycosidic bonds in glycogen and amylopectin. The resulting glucose syrup is a major ingredient in food manufacturing, and its properties depend heavily on the degree of hydrolysis, expressed as the D-glucose equivalent or DE value. A higher DE means more complete breakdown into individual glucose units. Corn syrup with a DE of 42 is commonly used in beverages, while maltodextrins with lower DE values serve different functional purposes in processed foods. From a nutritional standpoint, the glycemic index measures how quickly glucose raises blood sugar compared to pure glucose, which has an index of 100 by definition. Foods with high glycemic indices cause rapid spikes in blood glucose and insulin, which over time contributes to insulin resistance and metabolic syndrome. This is not controversial biochemistry, but it is relevant when considering why understanding glucose metabolism matters beyond the laboratory. The difference between eating a piece of fruit and drinking fruit juice is partly about the rate of glucose absorption, which is affected by fiber content and food matrix structure. Glucose is also used in medical settings as intravenous dextrose solutions for patients who cannot eat or need rapid carbohydrate delivery. The concentration matters here. A 5% dextrose solution is roughly isotonic, while higher concentrations like 10% or 50% are hypertonic and can cause vein irritation if not administered through a central line. I have seen cases where hypertonic dextrose was given through a peripheral IV and resulted in phlebitis, so the practical handling of glucose solutions requires attention to concentration and administration route, not just the chemistry.
Key Takeaways for Working with Glucose
Know the anomeric state of your glucose. Whether you are running an enzymatic assay, a fermentation, or a glycosylation reaction, the alpha or beta configuration affects the outcome. Check the product specifications from your supplier. Validate your measurement method. Colorimetric assays are convenient but prone to interference. If accuracy matters, cross-check with an alternative method like HPLC or enzymatic measurement with different chemistries. Store glucose solutions properly. Aliquot, freeze, and avoid repeated thawing. Degradation products accumulate slowly and affect results in ways that are hard to detect without proper controls.
Account for mutarotation in any polarimetric or kinetic measurement. Allow equilibrium or control the timing precisely. The chemistry of glucose is straightforward on paper. The complications arise in practice, and those complications are what separate reliable results from frustrating inconsistencies. Understanding the structural details, the measurement limitations, and the stability issues saves time and prevents errors that are otherwise difficult to trace.