Transcription Machinery: A Practical Breakdown
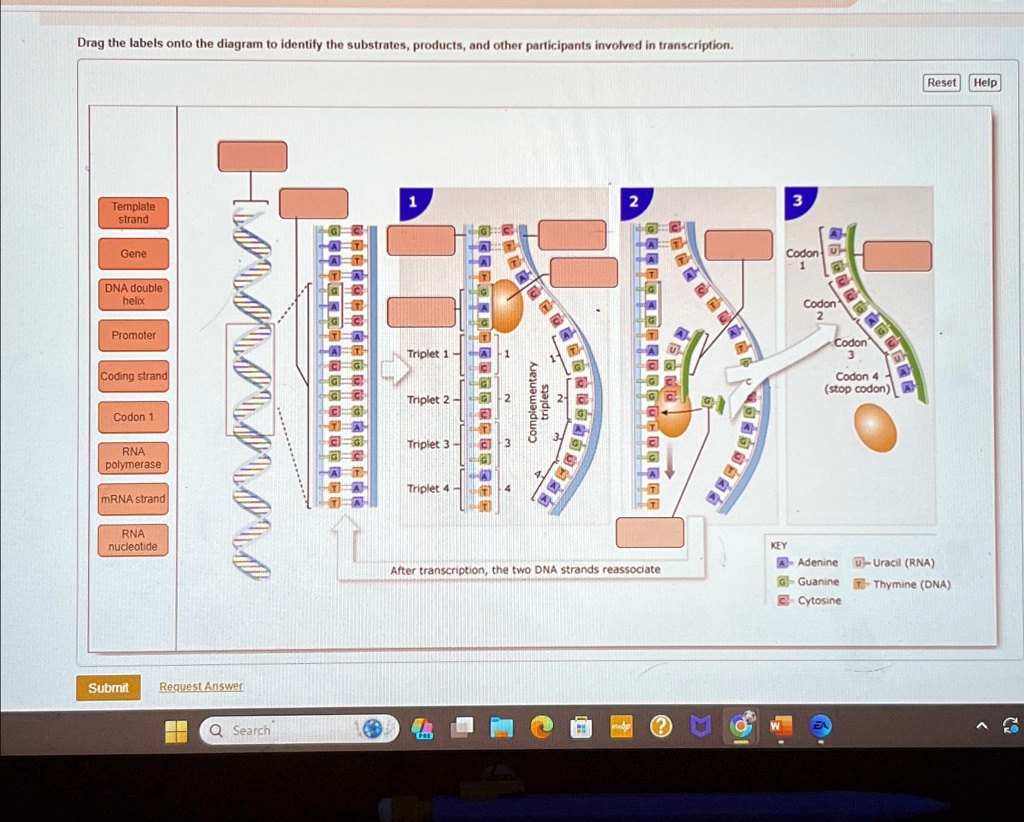
Most people learning molecular biology hit a wall when they try to actually understand transcription as a system rather than a diagram in a textbook. You memorize the steps, draw the arrow from DNA to RNA, call it a day. Then you try to work with it in practice and realize you have no idea what is actually happening at the molecular level. I spent three years in a lab before this clicked for me. Let me start with what actually powers the process because that is where most explanations get it wrong. ATP, GTP, CTP, and UTP are not just building blocks. They are both the substrate and the energy source in one molecule. Each incoming nucleoside triphosphate provides the free energy for phosphodiester bond formation through pyrophosphate release. You do not need a separate energy step. The high-energy bonds between the alpha, beta, and gamma phosphates are what drive polymerization forward. This is important because it means the process is inherently directional and irreversible under normal cellular conditions. The core enzyme in bacteria is RNA polymerase holoenzyme, which is a five-subunit core plus a sigma factor. In eukaryotes, you have three distinct RNA polymerases. Pol II handles mRNA, Pol I handles ribosomal RNA, and Pol III handles tRNA and other small RNAs. Each one has different promoter requirements and different regulatory mechanisms. You cannot substitute one for another without redesigning your entire system.
I ran into a specific problem once where my in vitro transcription reactions were producing mostly truncated products instead of full-length RNA. I spent two days troubleshooting before I realized the magnesium concentration was slightly too low. The optimal range for MgCl2 in these reactions is 6 to 10 millimolar, and my stock solution had degraded over time. I replaced it and got clean full-length product in the next run. This kind of issue is easy to miss because the reaction still produces RNA, just not the right amount of it. You have to actually check your reagent concentrations periodically. Substrates are straightforward if you understand what you are working with. You need ribonucleoside triphosphates, not deoxy versions. Using dNTPs instead of NTPs will give you nothing because DNA polymerase does not recognize them as substrates for RNA synthesis, and RNA polymerase rejects them on steric grounds. The 3 prime hydroxyl group on the ribose is also essential. If you are doing something like capped RNA synthesis or modified nucleotide incorporation, you need special substrates that are compatible with the polymerase active site. Products depend entirely on which polymerase and which template you are using. Bacterial RNA polymerase can produce transcripts of several kilobases without falling off. Eukaryotic Pol II typically produces transcripts in the same range but requires capping, splicing, and polyadenylation signals for proper maturation. The raw product coming out of the polymerase is just a single-stranded RNA chain. Everything else is post-transcriptional modification.
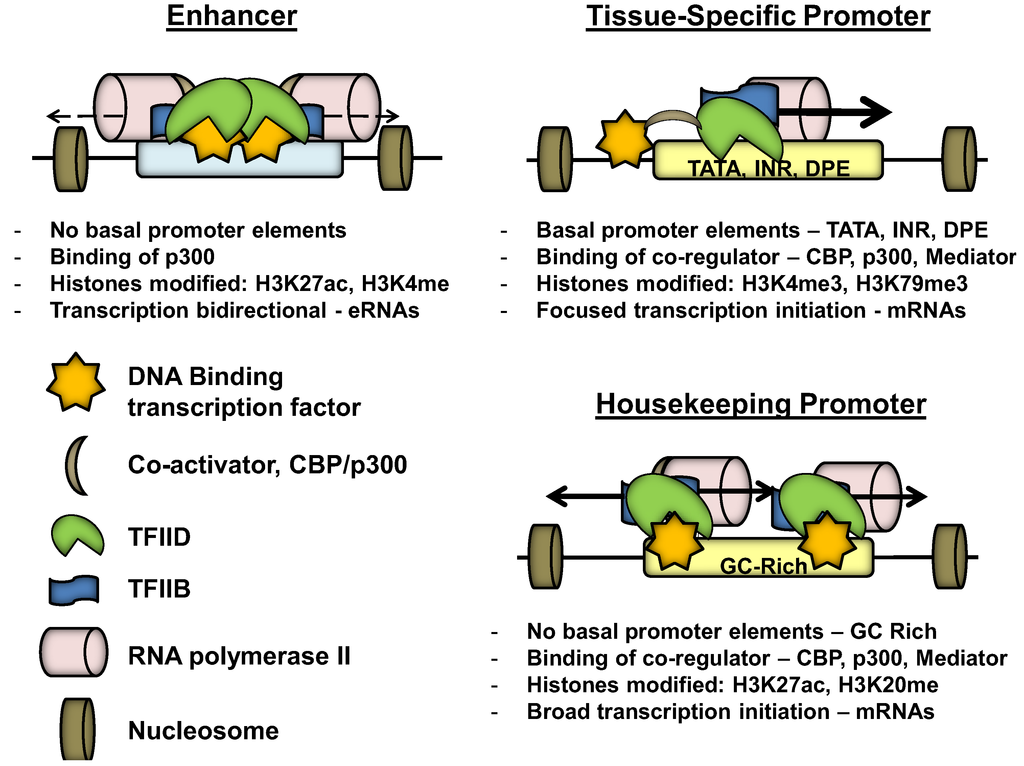
The supporting cast is where transcription gets complicated. Transcription factors are not optional accessories. Without them, most genes do not get transcribed at detectable levels. In bacteria, sigma factors determine promoter specificity. Different sigma factors redirect the RNA polymerase to different sets of genes under different conditions. Sigma 70 is the housekeeping factor. Sigma 32 activates heat shock genes. When the cell temperature rises, sigma 32 becomes more stable and outcompetes sigma 70 for binding to the core enzyme. This is a direct regulatory mechanism, not a secondary effect. In eukaryotes, the general transcription factors form a pre-initiation complex at the promoter before Pol II even arrives. TFIIA, TFIIB, TFIID, TFIIE, TFIIF, and TFIIH each have specific roles. TFIID recognizes the TATA box through its TBP subunit. TFIIB bridges TBP and Pol II. TFIIH has helicase activity that unwinds the DNA and kinase activity that phosphorylates the Pol II C-terminal domain. Without that phosphorylation event, the polymerase cannot transition from initiation to elongation. It just sits there stuck. Mediator is another critical component that beginners often overlook. It is a massive multi-subunit complex that physically connects gene-specific transcription factors bound at enhancers to the basal transcription machinery at the promoter. Without Mediator, most regulated transcription does not happen. It acts as a molecular bridge and a signaling hub simultaneously. The complexity here is why eukaryotic gene regulation is so much harder to model than prokaryotic systems.
Get the Full Details

Chromatin structure is another layer that completely changes the transcription landscape. DNA wrapped around histones is not accessible to polymerase or transcription factors. You need chromatin remodeling complexes and histone modifying enzymes to open up the structure before transcription can begin. Histone acetylation generally promotes transcription by neutralizing the positive charge on histones and weakening their grip on DNA. Methylation can go either direction depending on which residue is modified and how many methyl groups are added. This is not a simple on-off switch. I encountered a case where adding more transcription factor to a reaction did not increase output. The template DNA was in a plasmid with tight supercoiling, and the polymerase was stalling well before reaching the end of the gene. Adding topoisomerase to the reaction relaxed the supercoils and increased full-length product yield by roughly fourfold. This is a practical example of why understanding the physical state of your template matters as much as the biochemical components. Common pitfalls in transcription work include nuclease contamination, which will chew up your product. RNases are everywhere and extremely stable. Using DEPC-treated water and fresh reagents helps but does not solve everything. The biggest issue is usually inadequate template quality. Supercoiled plasmid DNA transcribes more efficiently than linearized DNA for some systems, but circular templates can cause read-through issues where the polymerase continues past your desired sequence. Linearized templates give cleaner boundaries but may reduce overall yield depending on the system.
Another issue is incomplete removal of template DNA from your final RNA product. If you are doing downstream applications like RNA-Seq or functional assays, residual DNA can interfere. DNase treatment usually handles this, but you need to inactivate or remove the DNase afterward or it will degrade your template in subsequent reactions. The practical takeaway is that transcription is not a simple linear process. It involves coordinated assembly of multiple protein complexes, energy expenditure from nucleotide hydrolysis, chromatin remodeling in eukaryotes, and extensive regulation at every step from initiation to termination. Understanding the individual components helps, but the real insight comes from seeing how they interact under actual experimental conditions. Theoretical knowledge gets you so far before you hit the bench and find out what actually works. If you are setting up an in vitro transcription system, start with a well-characterized template and a commercial RNA polymerase kit. T7, T3, and SP6 phage polymerases are the standard workhorses because they are single-subunit enzymes that recognize specific promoters and do not require additional factors. They produce high yields of RNA in short reaction times, typically 1 to 2 hours at 37 degrees Celsius. From there you can add complexity by incorporating modified nucleotides, adding cap analogs, or switching to eukaryotic systems that require Pol II and all the general transcription factors.
For cellular transcription studies, the variables multiply quickly. You are dealing with endogenous polymerases, chromatin context, regulatory element positioning, and feedback loops that adjust everything based on cellular state. This is why molecular biology research in this area relies heavily on techniques like ChIP, RNA-Seq, and reporter assays rather than simple biochemistry. The system is too complex to reduce to a test tube reaction without losing critical regulatory information. There is no single resource that covers all of this thoroughly because the field moves fast. Papers on transcription mechanisms come out regularly, and new details about Mediator structure, chromatin remodeling, and elongation control are still being published. Staying current means reading the primary literature and keeping up with reviews in journals like Molecular Cell, Genes and Development, and Nature Structural and Molecular Biology. The bottom line is that transcription is a mechanistically understood process that remains experimentally challenging to manipulate precisely. You can get good results with standard protocols, but reproducing and optimizing those results requires attention to detail that goes beyond following a protocol sheet. The substrates, the polymerases, the factors, and the template quality all matter simultaneously. Neglect any one of them and the reaction will fail in ways that are not immediately obvious.