So You Want to Understand How Aerobic Biology Actually Works
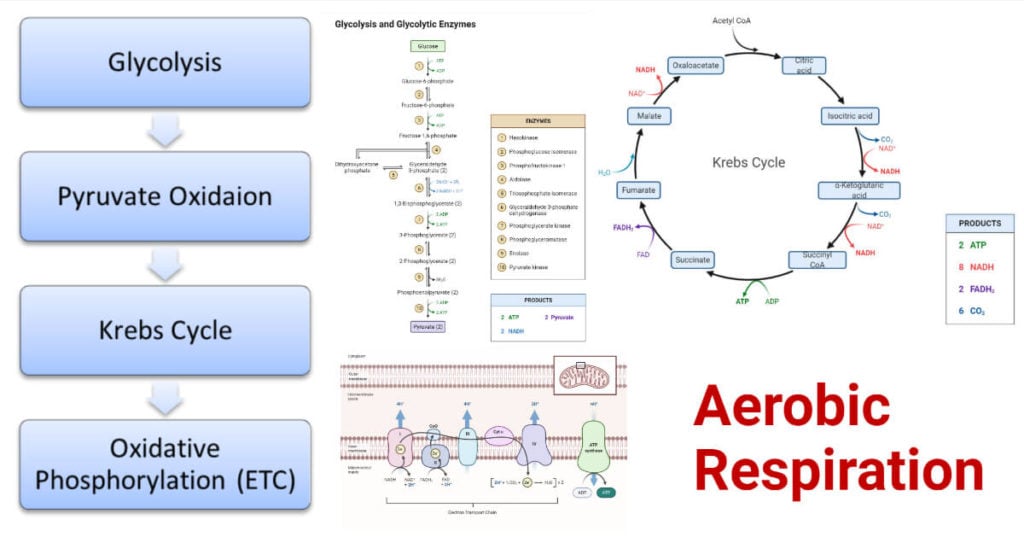
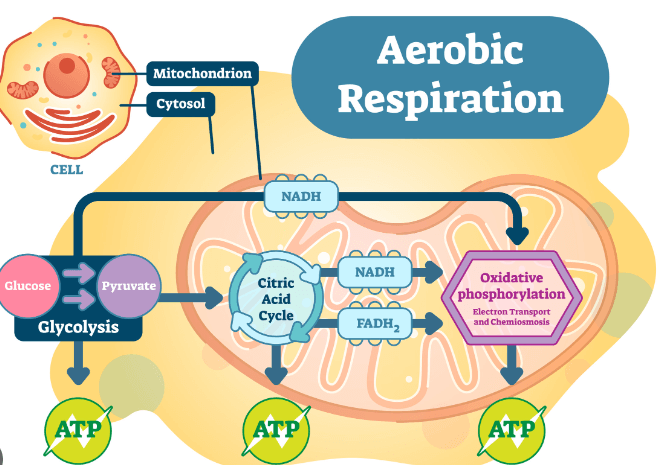
Oxygen is not just something we breathe in for drama. It is the final electron acceptor in a chain that powers nearly everything you find alive that has a nucleus worth studying. If you are trying to wrap your head around The Life Of Oxygen Understanding Aerobic Biology Definition, you are really looking at how cells extract energy from fuel using an oxidative process that would be impossible without O2 hanging around at the end of the line. Here is the thing most textbooks gloss over: aerobic biology is not about oxygen doing most of the heavy lifting directly. Oxygen sits at the bottom of the electron transport chain waiting. The real work happens way upstream, in glycolysis and the citric acid cycle, where electrons are pulled off carbon and shoved onto carriers like NAD+ and FAD. Those carriers then drop their cargo off at complexes I through IV embedded in the inner mitochondrial membrane. The energy released by those electrons falling down the redox gradient is what pumps protons across that membrane, building up a gradient that ATP synthase uses to make ATP from ADP and phosphate.
The Life Of Oxygen Understanding Aerobic Biology Definition
Breaking it down further, the definition rests on three interconnected processes that occur in sequence. Glycolysis splits glucose into two pyruvate molecules in the cytoplasm, netting two ATP and two NADH. Pyruvate then enters the mitochondrion and gets converted to acetyl-CoA, releasing one CO2 per pyruvate. The citric acid cycle runs through eight enzyme-catalyzed steps, producing three NADH, one FADH2, one GTP (convertible to ATP), and two more CO2 per acetyl-CoA. The electron transport chain and oxidative phosphorylation take all those reduced carriers and run them through four protein complexes, ultimately combining electrons with oxygen and protons to form water. I spent several semesters in grad school troubleshooting why certain cell cultures were dying despite having plenty of glucose in the medium. The problem turned out to be that the lab used fetal bovine serum batches with inconsistent lactate dehydrogenase activity, which meant some batches were generating far more pyruvate than expected and pushing the TCA cycle into a state where NADH was backing up. The cells were technically aerobic, but they were functionally starved because the electron transport chain had nowhere to send electrons. Adding a small amount of exogenous ascorbate to indirectly regenerate NAD+ from the backlogged ubiquinone pool fixed the culture viability. That told me a lot about how fragile the aerobic definition actually is in practice. What people routinely miss is that the stoichiometry of aerobic respiration is not a clean integer. The P/O ratio — how many ATP you get per oxygen atom consumed — has shifted over the decades as measurement techniques improved. Older textbooks will tell you three ATP per NADH and two per FADH2, giving you a theoretical yield of 36 or 38 ATP per glucose. Modern measurements put it closer to 2.5 and 1.5 respectively, for a total yield around 30 to 32 ATP. The difference comes from proton leak across the inner membrane, the cost of shuttling NADH from the cytoplasm into the mitochondrion via the malate-aspartate or glycerol-3-phosphate shuttle, and the fact that some proton gradient is used for transporting phosphate and ADP across the membrane, not just driving ATP synthase.
Another counter-intuitive point: aerobic organisms can and do run without fully functional mitochondria in certain tissues. Red blood cells lack mitochondria entirely and rely exclusively on anaerobic glycolysis. Some cancer cells, the Warburg effect, prefer fermentation even when oxygen is plentiful. This is not a biological failure mode. It is a strategic tradeoff where rapid ATP production rate matters more than efficiency. Glycolysis alone produces ATP about 100 times faster per glucose molecule than oxidative phosphorylation, even though it gets you only 2 ATP instead of 30. Your muscles during a sprint are running a similar logic, and that is why you burn through glycogen stores in minutes during high-intensity effort. There are also conditions where aerobic biology simply stops being useful. Deep sediments, anoxic water columns, and the guts of certain organisms have environments where the redox potential is too low for oxygen to serve as an electron acceptor. In those places, organisms switch to alternative terminal acceptors like nitrate, sulfate, or carbon dioxide. Sulfate-reducing bacteria for instance generate far less energy per electron pair than aerobic respiration, which is why those ecosystems have much slower growth rates and lower biomass turnover. If you are modeling any kind of biogeochemical cycle, assuming aerobic conditions where they do not exist will throw your energy yield calculations off by orders of magnitude. The bottleneck most people encounter when studying this topic is that the individual pathways are easy to memorize but the connections between them are not obvious. The link between the electron transport chain and the citric acid cycle is actually the availability of oxidized carriers. If NAD+ runs out, the TCA cycle stops regardless of whether you have ample oxygen or glucose. That is why the aerobic definition is fundamentally about the regeneration of those carriers through oxygen-dependent electron transport, not just about oxygen presence in isolation.
Get the Full Details
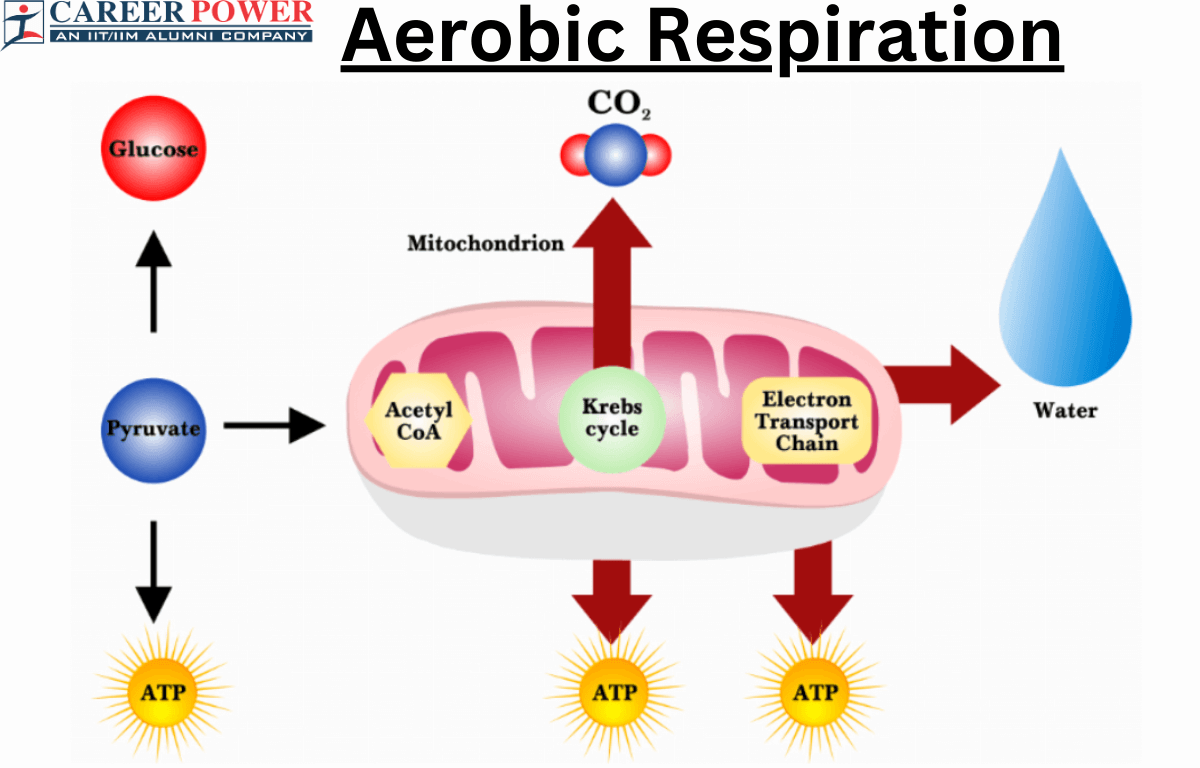
If you want a practical way to internalize this, trace a single carbon from glucose all the way to CO2 and follow its electrons through every carrier and complex. Do it on paper once without looking at a diagram. You will notice things like how complex II feeds into the same quinone pool as complex I but bypasses the first proton-pumping step, which is why FADH2 yields less ATP. You will also see that oxygen does not interact with any single complex until complex IV, where four electrons reduce one O2 molecule to two H2O molecules while pumping four additional protons. The takeaway is that aerobic biology is less a single process and more a dependency chain. Oxygen is the keystone, but the whole structure collapses if any upstream step fails, and it operates at a fraction of its theoretical efficiency due to real-world membrane physics. Understanding that gap between the textbook numbers and the actual cellular output is what separates someone who can recite the Krebs cycle from someone who actually understands what aerobic life does.