Speciation Isn't What Most People Think It Is
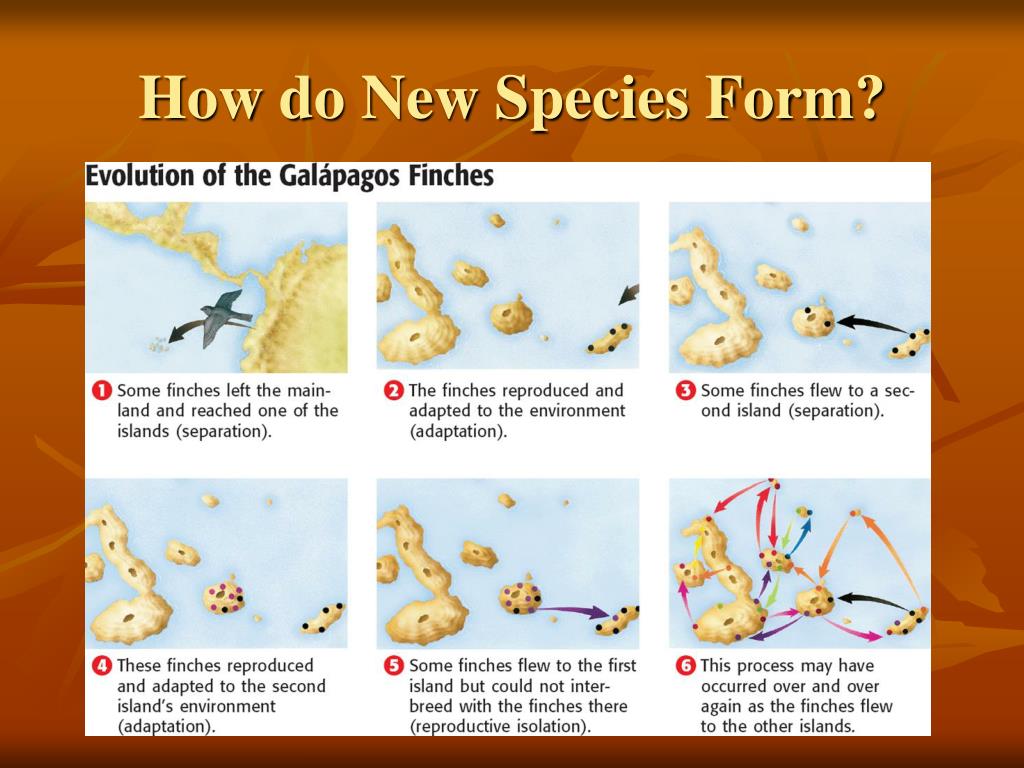
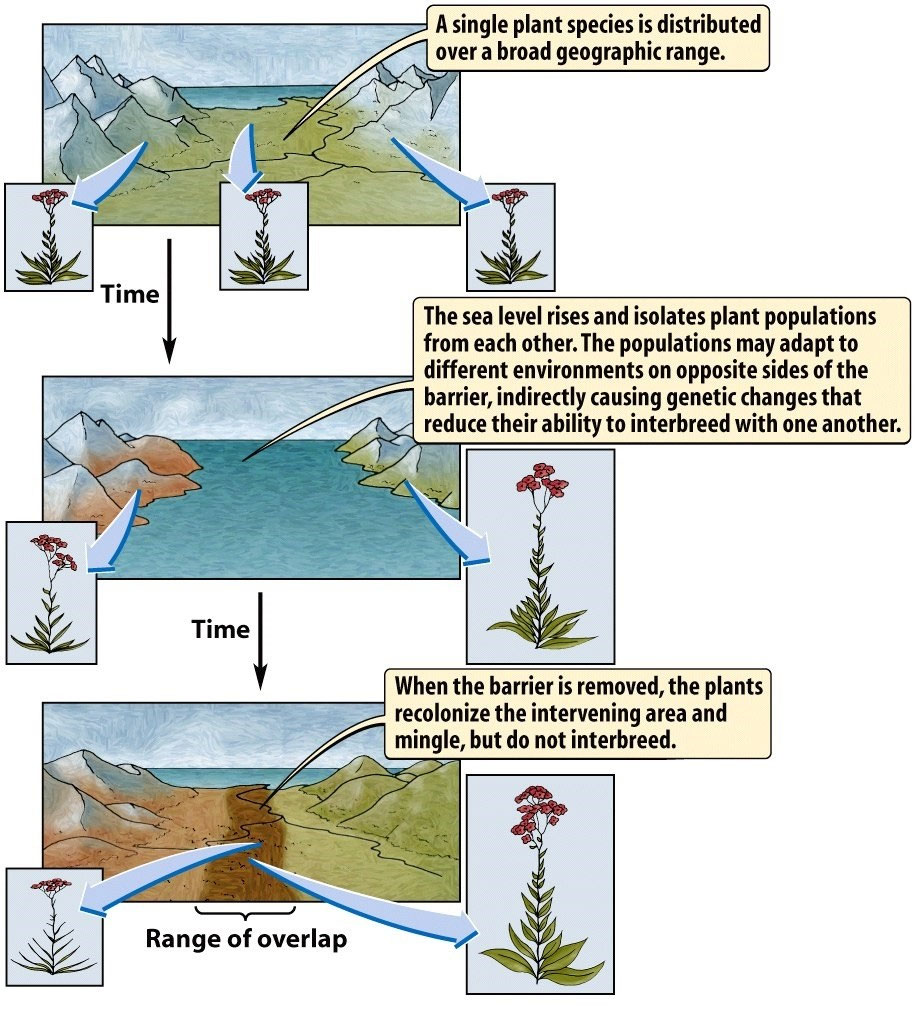
The formation of new species through evolutionary mechanisms is one of the most misunderstood topics in biology, and not just because textbooks oversimplify it. When you actually look at the data — phylogenetic trees, genomic comparisons, field observations over decades — the picture that emerges is messy and full of exceptions. I spent years working in systematics and population genetics, and even after all that time, I still get tripped up by how much variation exists between different speciation models. At the core, speciation requires reproductive isolation. That's the non-negotiable part. Two populations need to stop exchanging genes, and once that happens consistently enough, they diverge into separate species. The mechanisms that create that isolation fall into a few categories, and understanding which one is operating in any given case changes how you'd actually study it. Allopatric speciation is the baseline model. A geographic barrier — mountain range, river, ocean — splits a population. Over time, genetic drift and independent selection pressures push the two groups apart. This is the most common form and the one most textbooks lead with. But here's the thing most people miss: geographic isolation alone doesn't guarantee speciation will happen. You can have two populations separated for millions of years that still haven't diverged reproductively. I saw this firsthand with certain freshwater fish in the Amazon basin, where river course changes created isolated pools that should have produced distinct species based on time alone. Instead, the fish remained virtually identical genetically. Stasis isn't rare — it's the default in many environments where selection pressures stay consistent.
Peripatric speciation is a subset of allopatric speciation but worth treating separately because the dynamics are different. A small subpopulation gets isolated at the edge of the main range. The small population size means genetic drift dominates over selection, which can produce rapid divergence. This is the founder effect in action, and it explains why island biogeography is such a rich source of speciation examples. The problem is that peripatric speciation is extremely hard to confirm in practice. By the time you find evidence of a small founding population, that population has usually expanded and the original demographic signal is gone. You're often left with inference rather than direct observation. Parapatric speciation occurs when populations are adjacent rather than fully separated. There's a gradient — a cline — across the landscape, and divergence happens despite some gene flow between the populations. This is less common than allopatric speciation but more common than people assume. The classic example involves soil tolerance in grasses near mining sites. Plants on contaminated soil evolve tolerance through selection, and this tolerance comes with a reproductive cost when crossing with non-tolerant plants from nearby normal soil. Over time, the two types repel each other genetically even though they're physically next to each other. The mechanism here is strong disruptive selection overcoming gene flow, and it's fragile. If the contamination gradient shifts or the selective pressure weakens, the whole process can reverse. Sympatric speciation is the most controversial model because it requires divergence without any physical barrier. The leading mechanism is ecological specialization — a subset of a population starts exploiting a different niche within the same geographic area. Apple maggot flies are the textbook case, shifting from hawthorn fruit to apple trees and evolving different mating times as a result. But sympatric speciation through polyploidy is far more straightforward and well documented, especially in plants. Whole genome duplication can instantly create reproductive isolation in a single generation. I've worked with several plant genera where polyploid species sit alongside their diploid relatives, and the hybrid zones between them are sharp and stable. The polyploid individuals are reproductively isolated from day one because their chromosome numbers don't match up during meiosis with the diploid population.
Here's something that isn't covered adequately in most introductions: the role of sexual selection in speciation. In cichlid fishes of the East African rift lakes, mate choice based on coloration has driven speciation faster than any ecological factor. Different male color morphs attract different female preferences, and this creates strong assortative mating within the same lake. The reproductive isolation here isn't geographic or ecological — it's behavioral. And it's reversible. If the visual environment changes, say from clear to turbid water, the speciation process can unravel because the visual cues females use to choose mates become unreliable. I ran into this exact problem when trying to reconcile molecular clock estimates with morphological divergence rates in certain cichlid lineages. The genetic data suggested older splits than the fossil and morphological record indicated, and sexual selection dynamics explained the discrepancy. Gene flow complicates everything. The traditional view treated speciation as a one-way process — isolation leads to divergence leads to new species. But modern genomic analysis shows that even after initial divergence, secondary contact and hybridization are common. Sometimes the hybrid zone stabilizes, sometimes one species absorbs the other, and sometimes reinforcement strengthens prezygotic barriers. The outcome depends on which isolating mechanisms are already in place and how strong selection against hybrids is. If you're actually trying to study or identify speciation in progress, start with genomic data rather than morphology. Phenotypic differences can be misleading — convergent evolution produces similar traits in unrelated lineages, and cryptic species look identical but are reproductively isolated. Genomic isolation metrics like FST values and ABBA-BABA tests can reveal gene flow patterns that morphology completely misses. I wasted months trying to classify certain moth populations based on wing patterns before sequencing showed we were looking at three cryptic species, not one variable one.
Get the Full Details

The practical bottleneck in speciation research isn't data collection anymore — it's interpretation. We can sequence genomes fast and cheap, but distinguishing whether genetic divergence represents incipient speciation, completed speciation, or just population structure requires careful statistical framework. Coalescent-based methods help, but they make assumptions about population size and migration rates that aren't always valid. Be cautious about papers that claim speciation events based on a single analytical method. Cross-validate with multiple approaches. There are also scenarios where speciation models break down entirely. Hybrid zones that persist for millennia without resolving, reticulate evolution in groups like oaks and sunflowers, and horizontal gene transfer in microbial systems all challenge the tree-like model of speciation. The biological species concept itself — defining species by reproductive isolation — works reasonably well for animals but falls apart quickly when you apply it to organisms that reproduce asexually or hybridize routinely. Alternative concepts like the phylogenetic species concept or the recognition concept each solve some problems while creating others. What actually matters in practice is being specific about which speciation model you're testing and which evidence you're using to support it. Vague claims about "speciation through natural selection" aren't testable. But specifying allopatric divergence with gene flow in a particular system and backing it with genomic, ecological, and temporal data is. The hidden forces driving speciation are real and well documented — genetic drift, selection, sexual selection, polyploidy, ecological opportunity — but their relative importance varies enormously between lineages and environments. The pattern isn't universal, and treating it like one is the most common mistake in the field.