Understanding The Three Domains And Why Your Textbook Got It Wrong
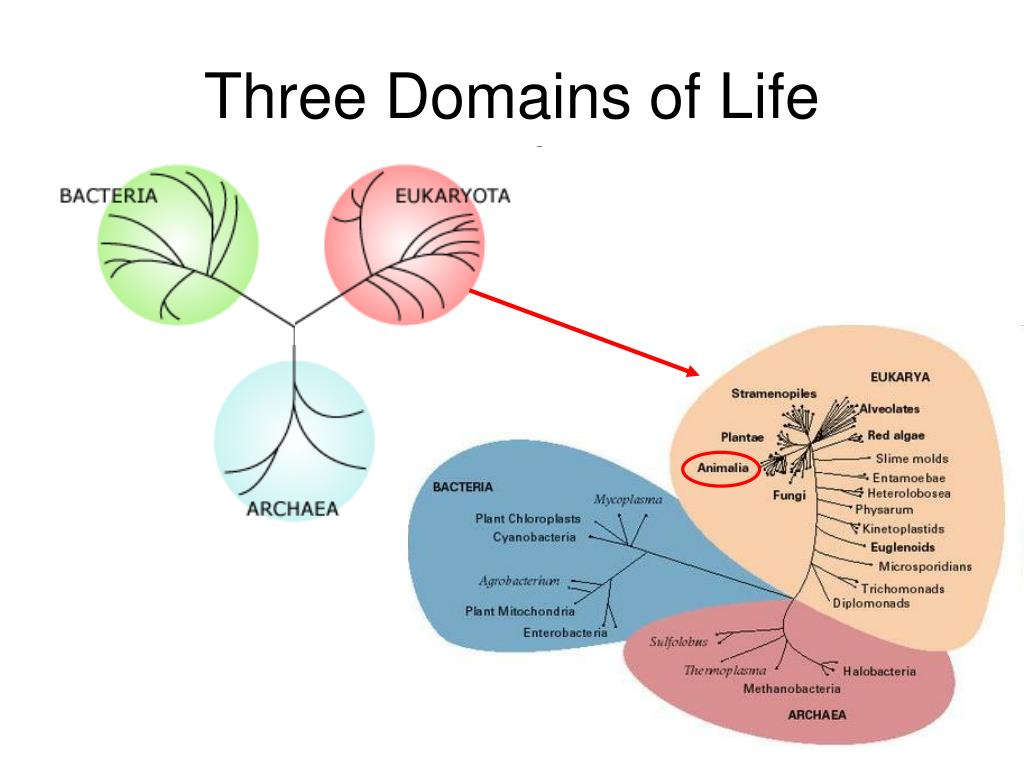
The three-domain system divides all cellular life into Bacteria, Archaea, and Eukarya. That sounds straightforward until you actually work with it in a lab. I spent years sequencing environmental samples from hydrothermal vents and hot springs, trying to place previously uncultured organisms into their correct domain. The real work starts when you realize 16S rRNA gene sequences from novel Archaea don't always cluster where you expect them to on a phylogenetic tree. You have to account for horizontal gene transfer, partial sequences, and PCR bias before you can say anything meaningful about what you're looking at. The three domains share core molecular machinery that points to a common ancestral cell, often called LUCA, or Last Universal Common Ancestor. The genetic code itself is nearly universal across all three domains, which tells us something important: this shared framework existed before the domains diverged, not after. Transfer RNA molecules use similar anticodon structures. Ribosomes across Bacteria, Archaea, and Eukarya all perform peptide bond formation through an RNA-based catalytic core, known as the peptidyl transferase center. That ribosomal RNA is conserved enough that you can align sequences from a human and a methanogenic archaeon and still see meaningful homology. But the similarities are where beginners trip up. People assume Bacteria and Archaea are more closely related to each other than either is to Eukarya because they both look like small single-celled organisms. That's wrong. Phylogenetic analyses consistently place Eukarya closer to Archaea, specifically within or sister to the Asgard archaeal lineage. Carl Woese originally proposed the three-domain system in 1977 based on ribosomal RNA sequence divergence, and while the framework has been refined significantly since then, the fundamental split between Bacteria on one side and the Archaea-Eukarya branch on the other has held up under increasingly sophisticated genomic analysis.
I encountered a specific problem a few years ago while working with a sediment sample from a deep-sea vent. We pulled out nearly complete 16S rRNA sequences that initially blasted against known Archaea databases but showed anomalous GC content and unexpected intron-like structures. Standard alignment tools misclassified them as bacterial contaminants because the reference sequences were too divergent. What we were actually looking at was a novel phylum within the Euryarchaeota that had undergone significant divergent evolution. The workaround was abandoning BLAST as the primary classification tool and instead using phylogenetic placement with pplacer or EPA-ng against a curated reference tree built from multiple domain representatives. That method accounts for branch length and evolutionary distance in a way that simple similarity searches don't. It also required running HMM profiles from the SILVA database rather than relying on raw sequence identity thresholds. The practical differences between the domains matter more than you'd think when you're actually doing biological work. Bacterial cell membranes use ester-linked fatty acids attached to glycerol-3-phosphate. Archaeal membranes use ether-linked isoprenoid chains on glycerol-1-phosphate. That's not a minor chemical distinction. Archaeal lipids form monolayer membranes in some hyperthermophiles, which is why organisms like Sulfolobus or Pyrolobus fumarii can survive above 100 degrees Celsius without their membranes melting apart. Bacterial and eukaryotic membranes simply cannot handle that kind of heat. You see this come up directly when someone tries to express an archaeal membrane protein in an E. coli system and the whole thing misfolds because the lipid environment is fundamentally incompatible. Translation mechanisms also diverge sharply. Archaeal translation machinery closely resembles the eukaryotic version. Their RNA polymerases are multi-subunit enzymes similar to Pol II, whereas bacterial RNA polymerase is structurally simpler. Antibiotics that target bacterial translation, like tetracycline or chloramphenicol, generally don't affect Archaea because the ribosomal targets differ enough. That's a practical consideration if you're ever running experiments with mixed cultures or environmental samples where you need to selectively inhibit one domain while studying another.
Eukarya are defined by the presence of a membrane-bound nucleus and organelles, which is the most obvious morphological distinction. But the endosymbiotic theory that explains mitochondrial and plastid origins is where the domains blur together. Mitochondria descended from an alpha-proteobacterial ancestor that was engulfed by an archaeal host cell. Most of that bacterium's genome moved into the host nucleus over evolutionary time, but the organelle retained its own circular DNA. Chloroplasts came later from a cyanobacterial endosymbiont. So every eukaryotic cell is literally a composite of organisms from at least two different domains operating inside one cellular boundary. That's not metaphorical. It's the literal molecular mechanism behind how complex life assembled itself. Here's the nuance that most introductions skip: the three-domain system is increasingly seen as incomplete by researchers working in the field. The alternative two-empire model proposed by William Martin and others argues that the domain tree is more of a network, with extensive early horizontal gene transfer blurring clean categorical boundaries. Some phylogenomic studies suggest that Eukarya didn't emerge from a single archaeal lineage but rather from a chimeric ancestor that combined archaeal and bacterial components in ways we're still trying to reconstruct. The Asgard archaea discovery in 2015 provided the strongest evidence yet for an archaeal host, but even that doesn't resolve every debate about the precise topology of the deepest branches. Another complication is the growing number of ultra-small bacteria and mini-cells discovered in subsurface environments that challenge what we consider typical domain characteristics. Organisms like the Candidate Phylum Radiation (also called DPANN) include some of the smallest known cells, many of which have reduced genomes and symbiotic dependencies that make standard cultivation and classification approaches fail. When I was classifying novel sequences from groundwater samples, I ran into several 16S rRNA reads that were too short and too divergent to place confidently. The solution was to use metagenome-assembled genomes (MAGs) rather than single-gene phylogeny, which gave enough contextual genomic data to make meaningful taxonomic assignments.
Get the Full Details

The cosmic heritage angle comes from the fact that the molecular machinery shared across all three domains is built from atoms forged in stars. The carbon in your DNA, the nitrogen in your amino acids, the phosphorus in your ATP, the iron in your cytochromes were all synthesized in stellar nucleosynthesis or supernova events. The ribosome, which performs the same basic chemical reaction in a bacterium, an archaeon, and a human, is made of RNA and protein in roughly equal parts, and that ribozyme core is one of the most ancient molecular machines still in operation. You can see the same catalytic strategies in ribosomes from organisms that diverged over three billion years ago. Practical applications of this knowledge extend well beyond academic taxonomy. The study of extremophile Archaea has directly enabled biotechnology through enzymes like Pfu polymerase from Pyrococcus furiosus, which has become standard for high-fidelity PCR. The thermostability of these enzymes comes from the same membrane and protein adaptations that allow these organisms to live in conditions that would denature bacterial or eukaryotic proteins. Metagenomic surveys of extreme environments continue to yield novel enzymes and metabolic pathways that have industrial applications, from bioleaching to bioremediation. If you want to start exploring this yourself, the SILVA ribosomal RNA database and the GTDB (Genome Taxonomy Database) provide the most current and rigorously curated reference datasets for phylogenetic classification. GTDB has been particularly useful because it reclassifies organisms based on phylogenomic analysis of 120+ conserved protein markers rather than relying solely on 16S rRNA similarity, which resolves many of the ambiguities that plagued older classification systems. The All-Species Living Tree Project is also worth referencing for curated 16S-based classifications of cultured organisms.
The main limitation of working with the three-domain framework is that it's fundamentally a human categorization system imposed on a continuous evolutionary process. Nature doesn't draw clean lines between domains. Horizontal gene transfer, endosymbiosis, and viral gene exchange create constant molecular borrowing that crosses domain boundaries. The system is useful as a working model but should not be mistaken for a reflection of discrete natural units. When your sequencing data doesn't fit neatly into one domain, that's usually a sign that evolution is doing exactly what it does, which is combining and recombining existing machinery in new configurations.