What Actually Moves Across a Cell Membrane
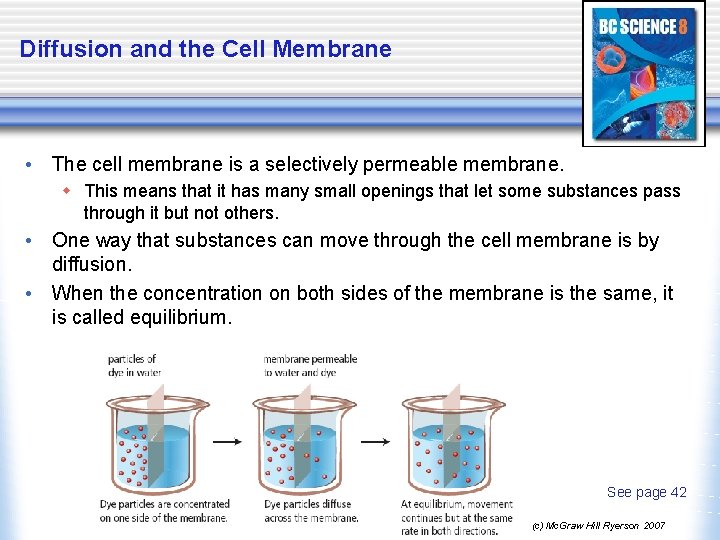
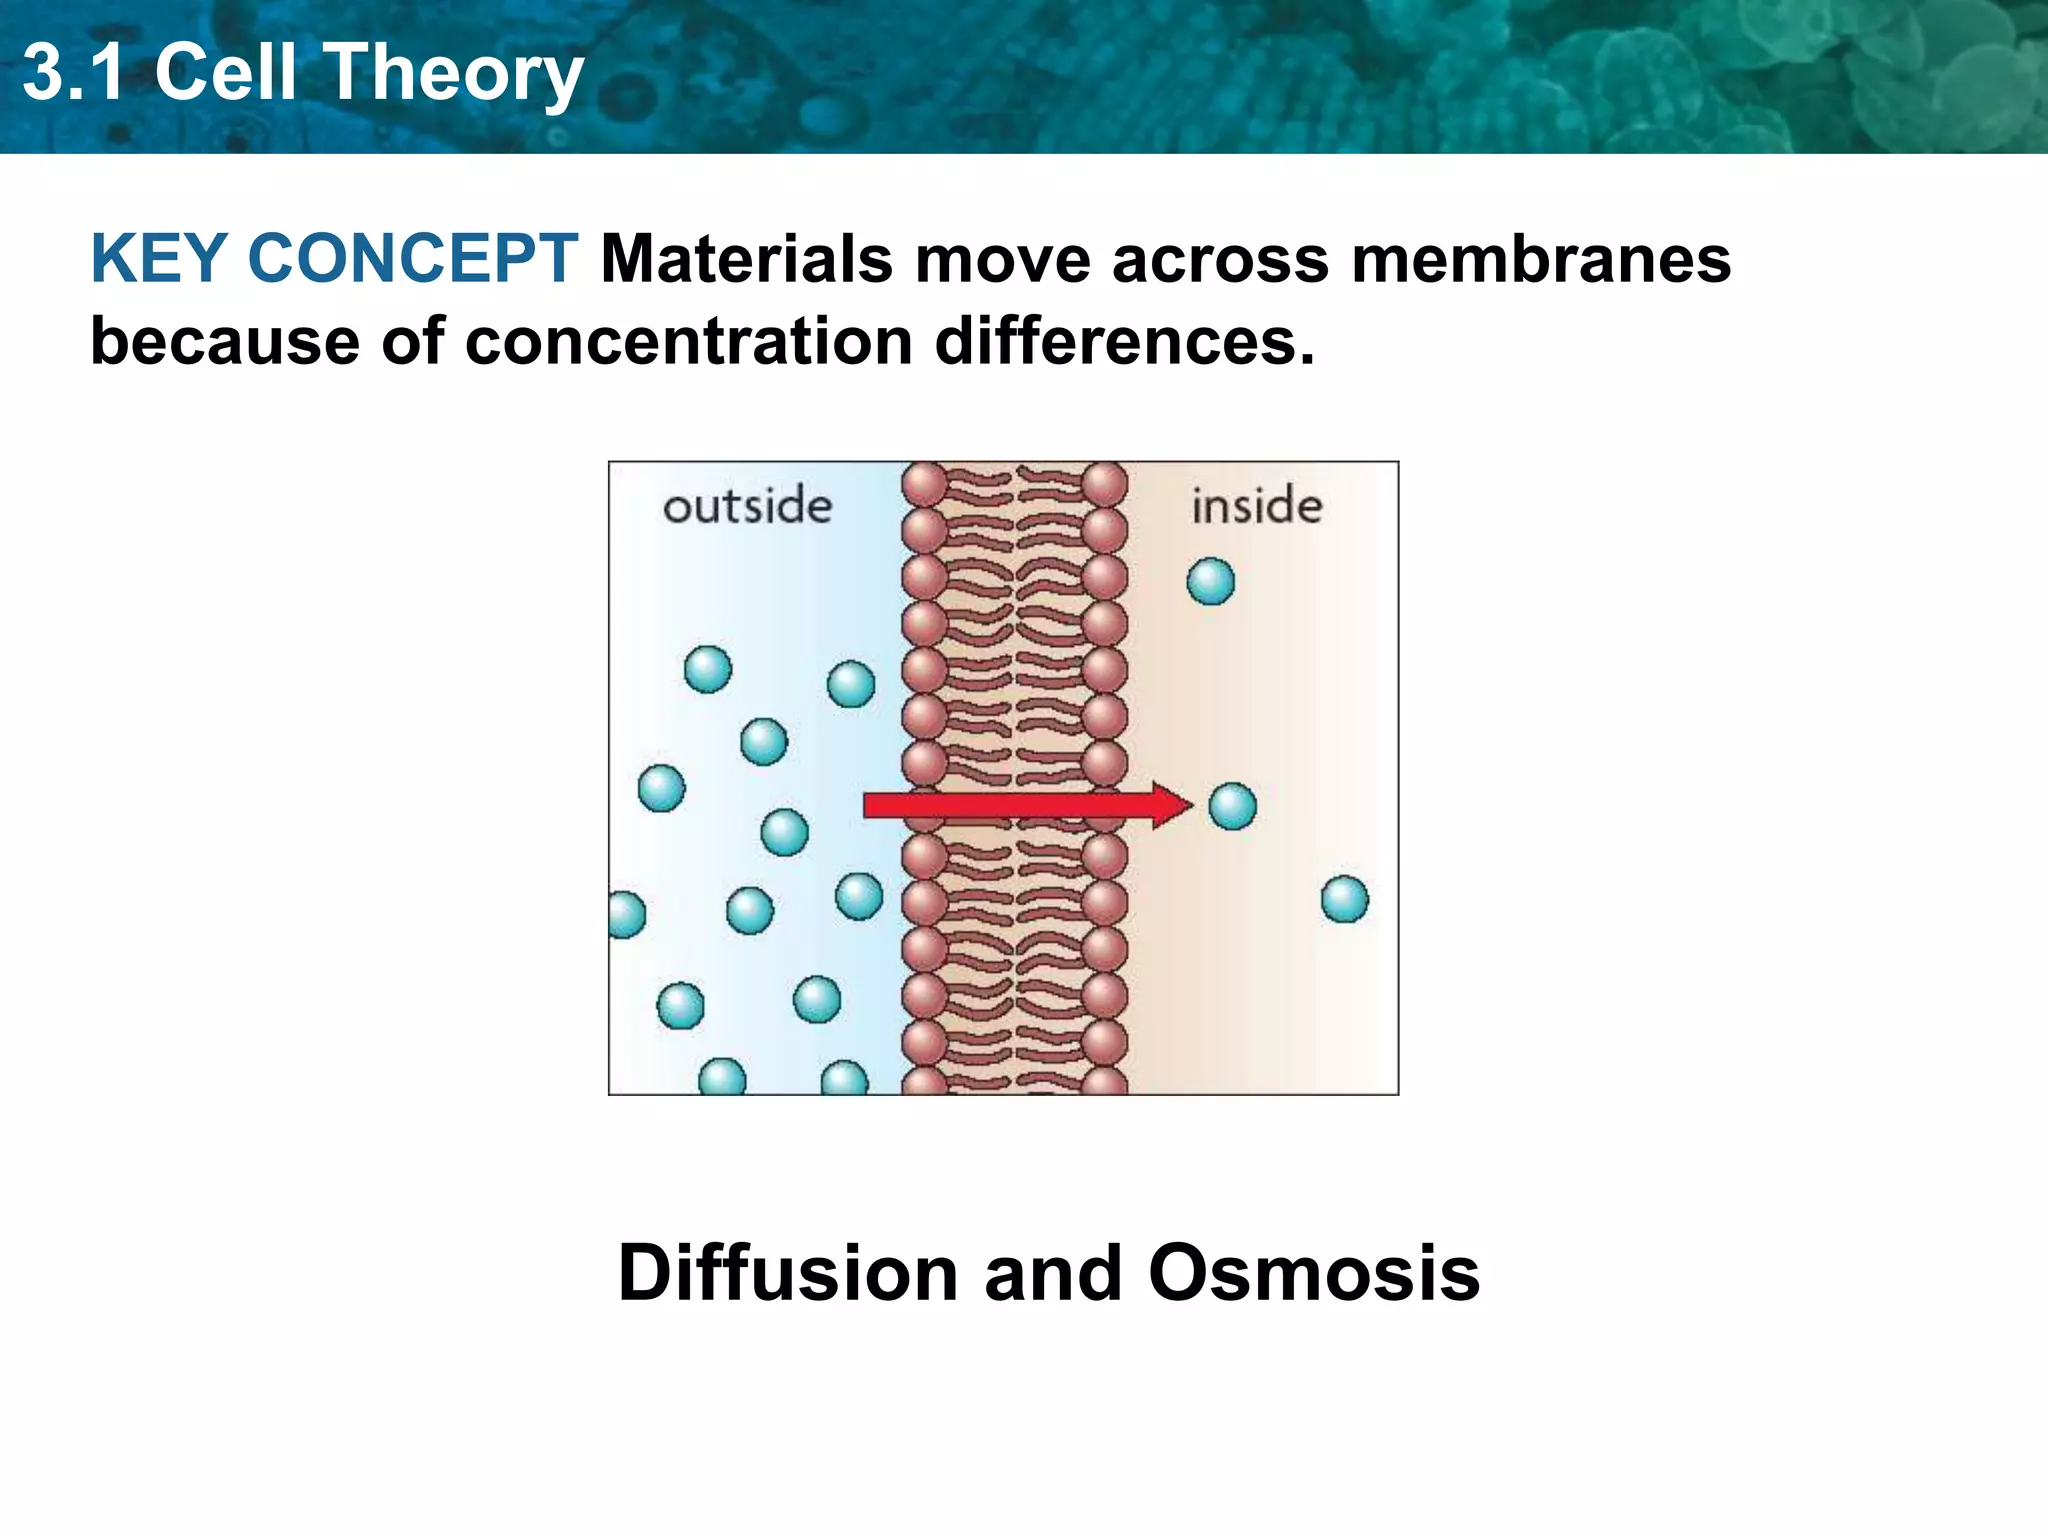
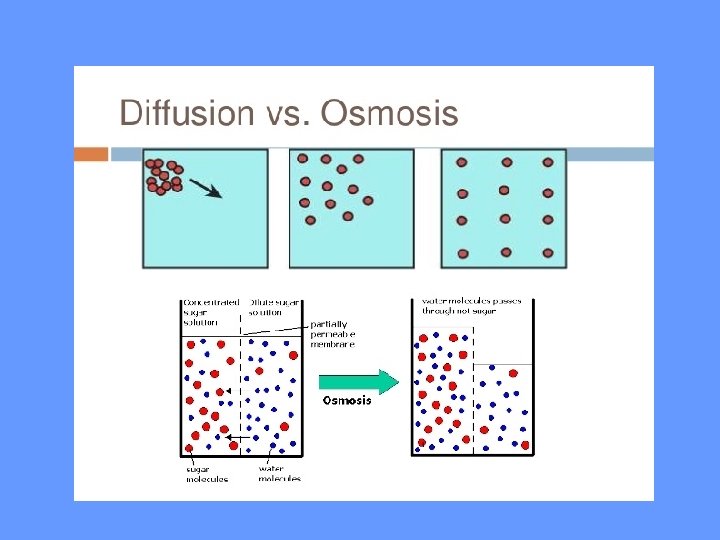
Most people learn osmosis and diffusion as two separate topics in biology class. They're not. They're the same physical process viewed from different angles. Diffusion describes the net movement of any solute or gas from high concentration to low concentration. Osmosis is specifically water moving across a semipermeable membrane toward the side with more dissolved particles. That's it.The Great Cell Conundrum Unraveling The Mysteries Of Osmosis And Diffusion
The confusion comes from the way textbooks present these ideas in isolation, usually with diagrams of red blood cells shrinking in salt water and stopping there. Nobody explains what happens next, or why plant cells don't burst the same way, or what tonicity actually means beyond "salt water bad." I spent years working with cell culture and membrane transport assays, and the first thing I learned was that textbook diagrams lie by omission. A 0.9% saline solution isn't just "isotonic" because some book says so. It's isotonic to human blood because that specific concentration produces the same osmotic pressure as plasma. Change the temperature, change the ions present, and that number shifts slightly. Real labs account for this. Textbooks don't bother.
How to Think About Osmotic Pressure Without the Memorization Trap
Osmotic pressure follows the van 't Hoff equation: = iMRT. The i factor is the van 't Hoff factor, which accounts for how many particles a solute dissociates into. NaCl dissociates into two ions, so its effective osmolarity is roughly double its molar concentration. Glucose doesn't dissociate, so its osmolarity equals its molar concentration. This distinction matters enormously when you're preparing solutions for actual experiments. Here's a concrete problem I ran into repeatedly. You're culturing mammalian cells and need to prepare a hypertonic stress solution. Someone tells you to use 300 mM NaCl. You add it directly to your culture medium and the cells die within minutes. The reason: your medium already contains roughly 150 mOsm of salts. Adding another 300 mOsm worth of NaCl doesn't give you a 300 mOsm solution. It gives you something closer to 450 mOsm, which is far beyond what most adherent cell lines tolerate. The workaround was straightforward once I stopped treating the numbers as absolute and started calculating total osmolarity from every component in the medium. I switched to using sucrose for hypertonic adjustments since it doesn't cross the membrane and its osmotic contribution is purely from the added amount. That single change made my stress protocols reproducible instead of chaotic.
Diffusion Is Not Always the Fast Option
Beginners assume diffusion happens quickly and osmosis is slow. That's backwards in most biological contexts. Water crosses membranes through aquaporins at rates that can exceed 10^9 molecules per second per channel. Small nonpolar molecules like O2 and CO2 diffuse directly through the lipid bilayer without any protein help, and they do so remarkably fast because the membrane is only about 5 nanometers thick at the point of passage. Ions, however, are essentially stuck. They can't cross the hydrophobic core without a channel or transporter, and without those proteins the effective permeability drops to near zero. The counter-intuitive part is that cell size itself becomes a diffusion limitation. A neuron's axon can be over a meter long in humans. Diffusion alone would take days for a molecule to traverse that distance. The cell solves this with active transport mechanisms and cytoplasmic streaming, but the fundamental constraint remains. This is why large cells are rare and why multicellular organisms evolved circulatory systems rather than simply growing bigger cells.
Get the Full Details

Facilitated Diffusion Is Where Things Get Messy
Glucose transport through GLUT proteins is facilitated diffusion. It moves down the concentration gradient without ATP, but it saturates. At low glucose concentrations the transport rate increases linearly with concentration. Once all the GLUT carriers are occupied, the rate plateaus. This is Michaelis-Menten kinetics applied to a membrane protein, and it's the reason oral glucose tolerance tests work the way they do. Your intestinal epithelium can only absorb glucose so fast, regardless of how much sugar you consume. A common pitfall in experimental design is assuming that because something is "passive transport" it's unconstrained. It's not. Every carrier protein has a turnover rate, a maximum velocity, and a substrate specificity. SGLT1, the sodium-glucose cotransporter, moves glucose against its concentration gradient using the sodium gradient as fuel. That's secondary active transport, not facilitated diffusion, and confusing the two will get your experimental results wrong every time.
Why Plant Cells Don't Lyse in Hypotonic Solutions
Animal cells in pure water swell and burst because they have no structural resistance to turgor pressure. Plant cells have a cell wall made of cellulose that generates counter-pressure. As water enters the vacuole, the protoplast pushes against the wall, and the wall pushes back. The pressure potential increases until it balances the osmotic potential. At that point net water movement stops, even though the solution outside is still hypotonic. This is why a wilted plant recovers after watering instead of rupturing. The cell wall limits expansion to a defined maximum volume. Xylem vessels and root pressure illustrate the same principle at the tissue level. Root cells actively pump ions into the xylem, lowering the water potential inside the vessel. Water follows osmotically from the surrounding soil through the apoplast and symplast pathways. The resulting positive pressure can push water several meters upward without any energy expenditure at the destination. It's not enough for tall trees, which rely on transpiration pull as the primary mechanism, but it's a elegant demonstration that osmosis works at scale.
Practical Measurements and Common Errors
If you're trying to measure osmotic effects in a lab setting, freezing point depression osmometry is the standard method. It's reliable, relatively inexpensive, and doesn't require living cells. The instrument measures how much the freezing point of your sample is depressed relative to pure water, which correlates directly to osmolarity. A properly calibrated osmometer gives readings within ±5 mOsm/kg, which is sufficient for most cell culture applications. The error most people make is assuming that molarity and osmolarity are interchangeable. They're not. A 1 M solution of CaCl2 isn't 1 Osm. It's approximately 3 Osm because calcium chloride dissociates into three ions. When someone reports "isotonic solution" without specifying whether they mean osmolarity or molarity, you should ask for clarification before proceeding. I've seen protocols fail because a researcher prepared a "300 mOsm" buffer using a salt that dissociates into multiple ions and ended up with roughly 900 mOsm instead. Another practical issue is temperature dependence. Osmotic pressure is directly proportional to absolute temperature. A solution that's isotonic at 37°C won't be exactly isotonic at room temperature, though the difference is usually small enough to ignore in teaching labs. In precision work, like preparing intravenous fluids, temperature control matters and the manufacturing process accounts for it explicitly.