So You Need to Understand What Goes Into Cellular Respiration
The Fuel Of Life Understanding The Reactants Of Cellular Respiration
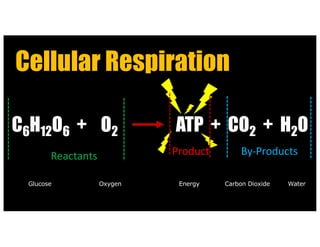
Most people learn the equation early and then forget how it actually works. C6H12O6 plus six molecules of oxygen yields six carbons dioxide, six waters, and roughly thirty ATP under ideal conditions. The reactants are glucose and oxygen. Everything after that is where the confusion starts. I spent a semester teaching introductory biochemistry and kept running into the same problems students had when they actually tried to trace the atoms through the pathway. A lot of them thought oxygen gets used up right away in glycolysis because the textbook simplifies things too aggressively. It doesn't. Glycolysis runs anaerobically. Oxygen only enters the picture at the very end of the electron transport chain as the final electron acceptor. If you tell someone oxygen is consumed during the first phase, you're already misleading them. Here's another thing that comes up constantly. Students assume glucose is the only fuel source. It isn't. Fatty acids feed into acetyl-CoA through beta-oxidation. Amino acids can be stripped of their nitrogen and funneled into the Krebs cycle at various entry points. But if we're talking about the classic reactants, yes, glucose and oxygen are the standard pair, and understanding why each matters separately is what actually helps you move past memorization.
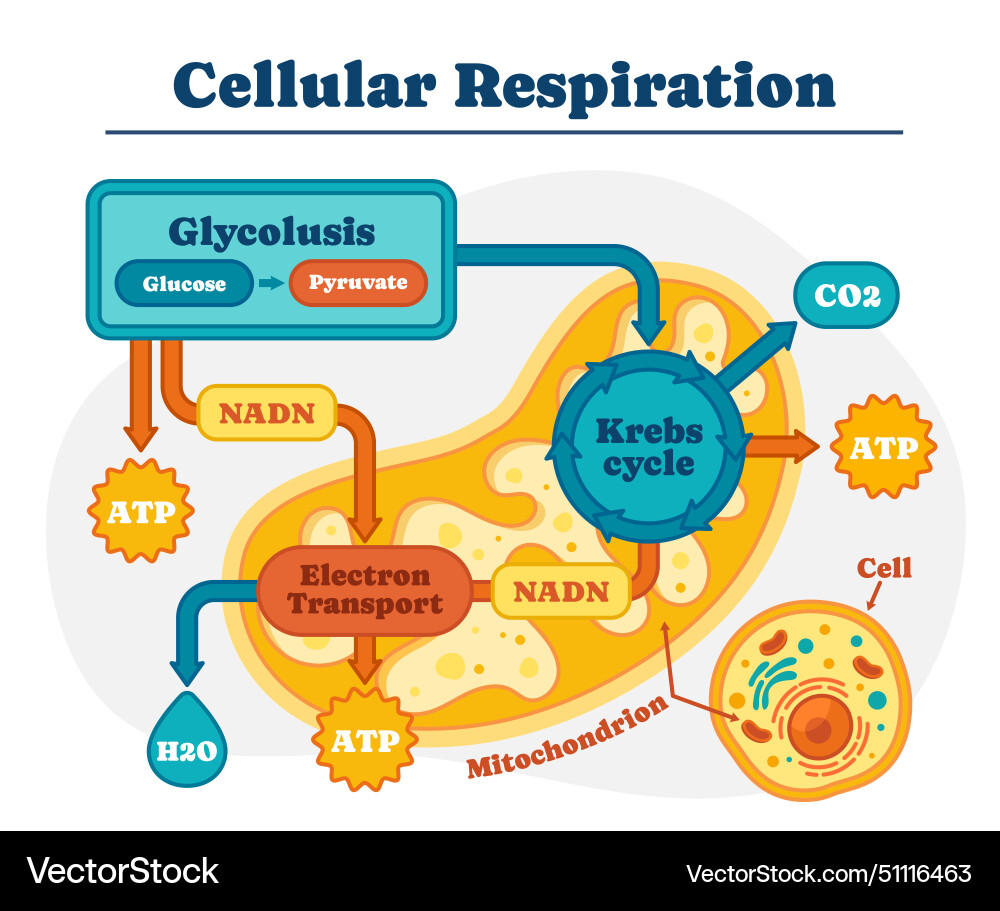
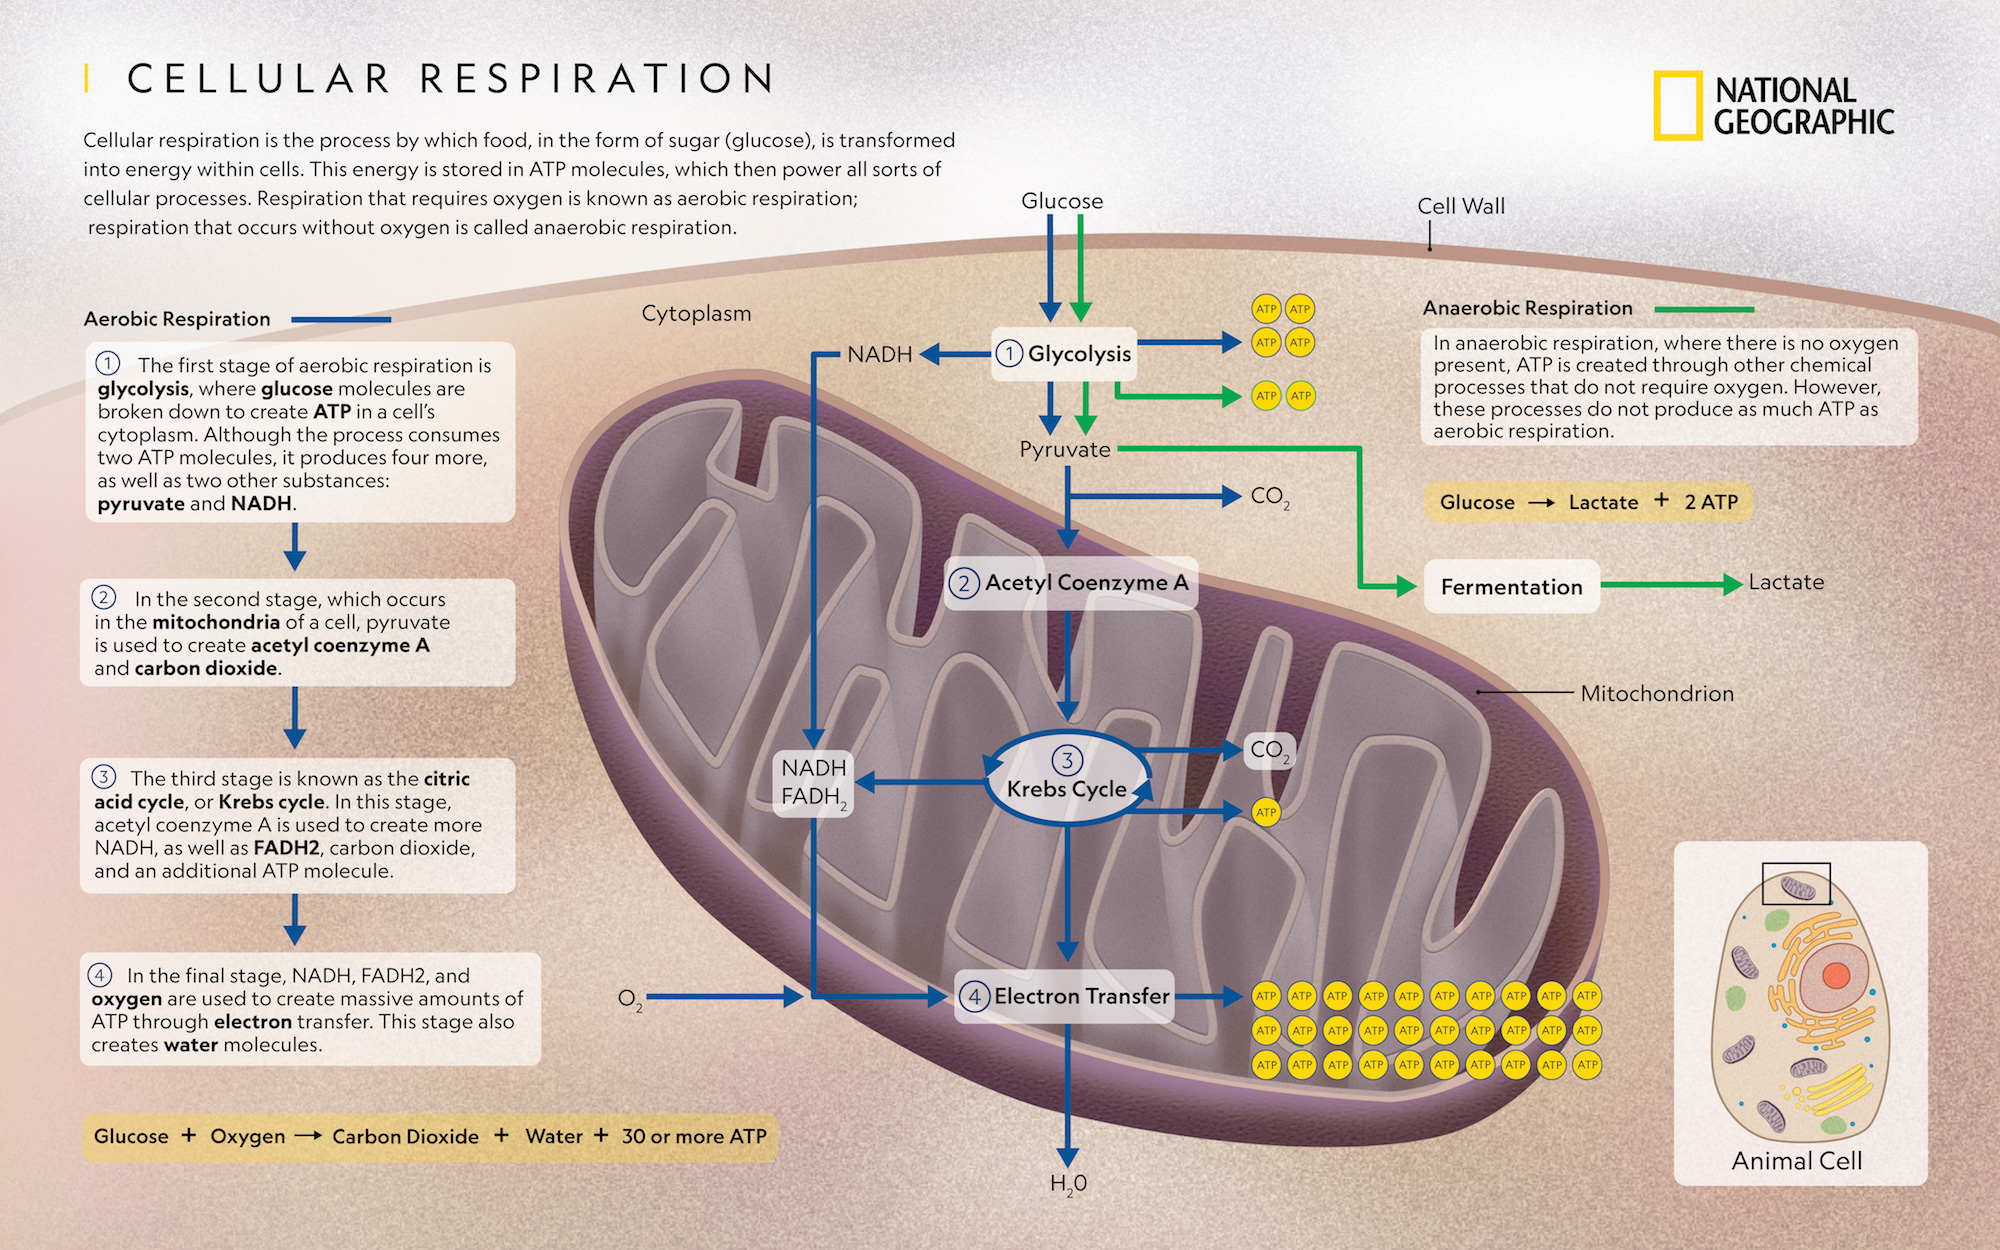
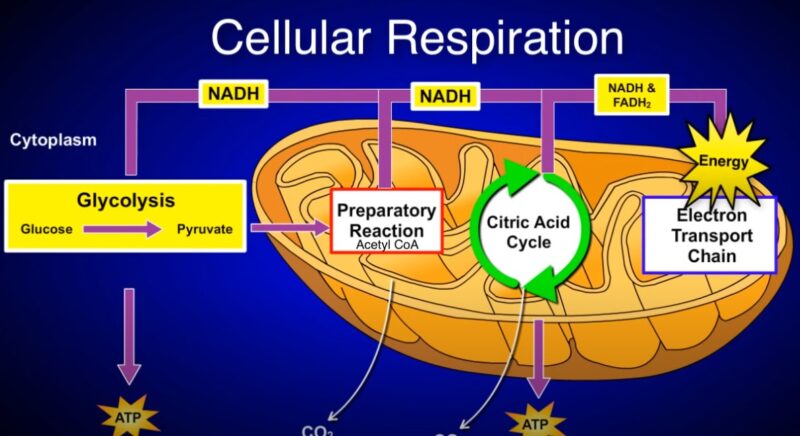
The glucose molecule gets broken down in the cytoplasm during glycolysis. That stage produces a net gain of two ATP and two NADH molecules. It also splits the six-carbon sugar into two three-carbon pyruvates. From there, the pyruvate moves into the mitochondrial matrix where it gets converted to acetyl-CoA, releasing one CO2 per pyruvate. The Krebs cycle then turns that acetyl group through a series of reactions, generating more NADH, FADH2, and another round of CO2. None of these steps actually require molecular oxygen directly. That's the part that trips people up most of the time. Oxygen's real job starts at Complex IV of the electron transport chain. It accepts electrons and combines with protons to form water. Without that terminal step, the entire chain backs up. NADH and FADH2 can't drop off their electrons. The proton gradient collapses. ATP synthase stops spinning. Aerobic respiration halts within seconds of oxygen deprivation because the system depends on keeping that electron flow moving continuously. I remember working with lab samples where the mitochondria were supposed to be respiring on pyruvate and malate as substrate pairs. We were measuring oxygen consumption rates with a Clark electrode, and the baseline was frustratingly low. Turned out the buffer solution had been prepared with tap water instead of deionized water, and the trace metals in the tap water were inhibiting Complex I activity. Ran the same experiment with freshly prepared deionized buffer and the rate jumped from about 20 nanomoles per minute to nearly 180. Small detail, massive impact on the readout. It's the kind of thing that doesn't show up in any textbook.
There's also a persistent myth about the ATP yield. Textbooks will tell you thirty-six or thirty-eight ATP per glucose molecule. The actual number in mammalian cells is closer to twenty-eight to thirty, and it varies between cell types. The shuttle systems that ferry NADH electrons from the cytoplasm into the mitochondria cost energy differently depending on whether you're using the malate-aspartate shuttle or the glycerol-3-phosphate shuttle. Brown fat uses a completely different mechanism with UCP1 that intentionally short-circuits the proton gradient to generate heat instead of ATP. So the yield isn't fixed. It depends on tissue, conditions, and which pathways are active at the moment. If you're trying to internalize how these reactants actually connect to the output, don't rely on the summary equation alone. Trace one carbon atom from glucose through to CO2. Watch where the hydrogens go. Follow the electrons through NAD+ and FAD to oxygen. The atoms don't disappear. They rearrange, and the energy difference between the bonds in glucose and oxygen versus the bonds in carbon dioxide and water is what gets captured in ATP. That energy gap is the whole point of the reactants. The biggest pitfall I see is treating this as a linear assembly line. It's not. It's a network of interconnected cycles with multiple entry and exit points, regulatory checkpoints at key enzymes like phosphofructokinase and isocitrate dehydrogenase, and feedback loops that respond to the actual energy state of the cell. ATP inhibits phosphofructokinase. When energy is abundant, glycolysis slows down regardless of how much glucose is available. The reactants are necessary but not sufficient. Regulation determines whether they get processed at all.
Get the Full Details

If you need a quick reference for the stoichiometry, the balanced equation remains the anchor. Six molecules of oxygen per glucose. Six molecules of carbon dioxide out. Six water molecules produced. Thirty-ish ATP depending on the shuttle and the tissue. Anything more precise than that requires specifying the exact conditions, and even then you're looking at ranges rather than fixed numbers. That's just how the biology works.