
Osmosis in Practical Terms
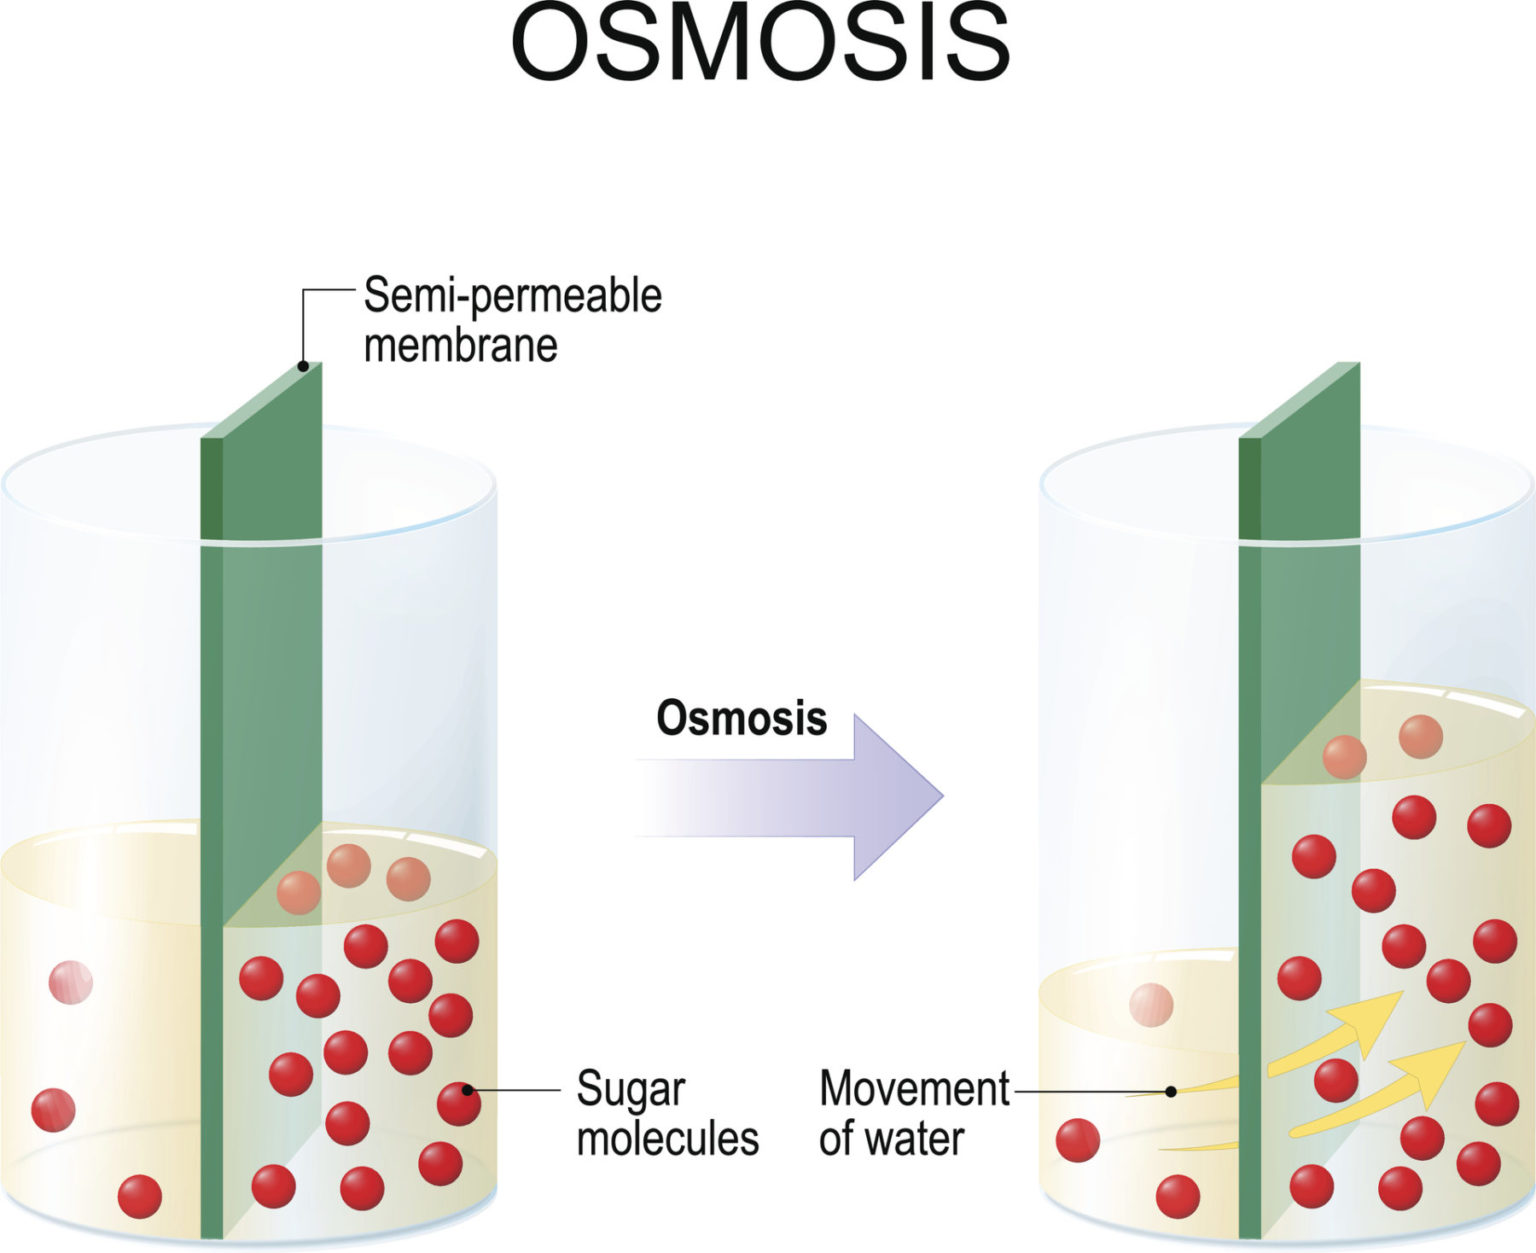
Osmosis is the passive movement of water across a semipermeable membrane from a region of lower solute concentration to a region of higher solute concentration. That definition you'll find in every textbook is correct but incomplete. In practice, osmosis is messy. Membranes vary. Solutes interact. Temperature shifts the whole balance. If you're doing anything beyond memorizing diagrams, you need to understand what's actually happening at the molecular level and how to predict when things go wrong. Water molecules are constantly moving. They don't sit still even when there's no net flow. The key is that water molecules move equally in both directions through the membrane's pores, but more water moves toward the side with higher solute concentration simply because there are fewer free water molecules on that side. Solute particles take up space and hinder water movement, so the net displacement of water is always toward the more concentrated solution. This is not water actively seeking out solutes. It's statistics. What drives osmosis is the difference in water potential between two solutions. Water potential (psi) combines solute potential and pressure potential. Pure water has a water potential of zero. Adding solute lowers it. Applying pressure raises it. Water moves from higher water potential to lower water potential until equilibrium is reached or external pressure prevents further movement.
The osmotic pressure formula, pi = iMRT, gives you the theoretical pressure needed to stop osmosis. Here i is the van't Hoff factor accounting for ion dissociation, M is molarity, R is the gas constant, and T is temperature in Kelvin. For a 0.1 M NaCl solution at 25°C, the osmotic pressure works out to roughly 4.9 atmospheres. That's significant. A single cell exposed to a solution of that concentration would lose water rapidly if its membrane couldn't handle the pressure differential. Don't confuse osmotic pressure with osmolarity. Osmolarity measures the total concentration of solute particles. Osmotic pressure is the force required to counteract osmosis. They're related but not interchangeable. When I was running plant physiology labs in grad school, students consistently mixed these up and their calculations were off by factors of two or three because they ignored the van't Hoff factor for ionic solutes.
What Actually Happens in Cells
Animal cells have no cell wall. Put a red blood cell in pure water and it swells and bursts. The membrane can only stretch so far before it fails. In a hypertonic solution, water leaves the cell and it shrivels. The range of isotonic conditions for human blood is narrow, roughly 0.9% sodium chloride or about 300 mOsm/L. Deviate by even 20% and you start seeing hemolysis or crenation. Plant cells behave differently because of the cell wall. Water entering the cell creates turgor pressure. The wall resists expansion and pushes back. At full turgor, the cell is firm but not damaged. That's why wilted plants perup again after watering. The cells were plasmolyzed, meaning the membrane pulled away from the wall as water left. Rehydration reverses this completely. I've seen field researchers lose entire samples of delicate tissue because they left specimens in a hypertonic buffer for too long before fixing. Plasmolysis is reversible in most cases but not if it's prolonged or extreme. Bacterial cells also have walls but the dynamics shift depending on whether you're dealing with Gram-positive or Gram-negative organisms. Their peptidoglycan layers differ in thickness and structure, which affects how they respond to osmotic stress. Salt curing works precisely because it creates an environment where most bacteria cannot maintain water balance and die or go dormant.
Get the Full Details

Common Pitfalls and What People Miss
One thing beginners consistently get wrong is assuming that any solute behaves the same way. Some molecules cross membranes easily. Urea passes through many biological membranes via facilitated diffusion. If you place a cell in a urea solution, water initially rushes out creating a hypertonic effect, but then urea enters the cell, reversing the gradient and causing the cell to swell. The observed effect changes over time. Sodium chloride does not cross easily, so the osmotic effect is sustained. This distinction matters enormously in IV therapy and cell culture work. Another overlooked factor is temperature. Osmotic pressure increases with temperature because water molecules move faster and collide with the membrane more frequently. A solution that's isotonic at room temperature might become hypotonic if warmed significantly. I learned this the hard way when running assays at different temperatures and seeing inconsistent cell volume measurements. The protocol specified 37°C but the stock solutions were prepared and stored at 22°C. The 15-degree difference shifted the osmotic balance enough to affect cell morphology noticeably. Membrane permeability is another variable textbooks barely touch. Real biological membranes are not ideal semipermeable barriers. They contain channels, carriers, and transporters that change effective permeability based on hormonal signals, pH, and other conditions. Aquaporins are water channel proteins that dramatically increase membrane permeability to water. Cells can regulate osmosis not just by changing solute concentrations but by inserting or removing these channels from the membrane. The kidney's collecting duct does this constantly under antidiuretic hormone control.
Practical Work With Osmosis
If you're working in a lab setting, the first thing to get right is your solution preparation. Use a calibrated balance, verify concentrations with osmolarity measurements rather than relying solely on calculated values, and account for temperature. When I switched to measuring osmolarity directly with a freezing point depression osmometer, my repeat failures dropped significantly. The calculated values and measured values rarely matched exactly, usually off by 5 to 15 percent depending on solute composition. For dialysis experiments or any setup involving artificial membranes, the membrane material and pore size determine which solutes pass and which don't. Cellophane dialysis tubing typically has a molecular weight cutoff around 12,000 to 14,000 Daltons. Smaller molecules diffuse out. Larger ones stay. But the rate depends on the concentration gradient, membrane surface area, and temperature. Stirring the external solution maintains the gradient by preventing local saturation near the membrane. I've seen people skip stirring and wonder why osmosis appeared to slow down after the first few minutes. It wasn't slowing down. The gradient was collapsing locally. When working with living tissues, the timing is critical. Osmotic effects can change cell volume within seconds to minutes depending on the gradient strength and membrane properties. Fixation stops the process immediately but can introduce artifacts if the fixative itself is not properly osmotic. Glutaraldehyde in a phosphate buffer is standard for electron microscopy, and the buffer must be isotonic or slightly hypertonic to prevent swelling artifacts. I once spent a week troubleshooting what I thought was a microscope alignment problem before realizing the tissue had been fixed in hypotonic buffer and the cells were swollen beyond recognition.
Where Osmosis Fails as an Explanation
Osmosis alone does not explain everything about water movement in biological systems. Active transport of ions creates the gradients that drive osmosis in the first place. The sodium-potassium pump consumes ATP to maintain the ionic imbalances that keep cells functional. Without active transport, osmosis would reach equilibrium and life would stop. The two processes are linked but distinct. Osmosis also doesn't account for bulk flow. When blood moves through capillaries, pressure-driven flow dominates over osmotic effects at the arterial end. Only at the venous end does osmotic pressure become the primary force pulling fluid back into the vessel. Starling forces combine hydrostatic and osmotic pressures to describe this balance. Ignoring the hydrostatic component gives you an incomplete picture. In plants, osmosis explains water uptake by root hairs but it cannot explain the ascent of sap to the top of a tall tree. Transpiration pull and cohesion-tension theory handle that. Osmosis contributes to root pressure, which can push water a few meters upward, but that's negligible in tall trees. Claims that osmosis alone moves water from roots to leaves are physically incorrect.

Understanding Tonometry and Osmolality Measurements
Freezing point depression is the gold standard for measuring osmolality in biological fluids. It works because any solute dissolved in water lowers the freezing point proportionally to the number of particles, regardless of their identity. One osmoles of any solute lowers the freezing point of one kilogram of water by 1.86°C. This is independent of solute type, which makes it far more reliable than methods that depend on chemical reactivity. Vapor pressure osmometry is an alternative for high-concentration samples where freezing point depression becomes less accurate. It measures the lowering of vapor pressure caused by dissolved solutes. Both methods give results in milliosmoles per kilogram (mOsm/kg), which is the standard unit in clinical and research settings. When I run quality controls on our osmometer, I use commercial standards at three levels: low, mid, and high. Acceptable variation is typically within 5 mOsm/kg of the target value. If readings drift outside that range, I check the calibration, clean the sample chamber, and verify the thermistor response. Maintenance is straightforward but often neglected until results become unreliable.
A Note on Misconceptions in Education
The diagram of a cell in hypotonic, isotonic, and hypertonic solutions appearing in every biology textbook is useful but oversimplified. Real cells adjust their internal solute content over time through regulatory volume mechanisms. Animal cells release ions and organic osmolytes when swollen and accumulate them when shrunk. Plant cells adjust osmolyte concentrations in response to environmental osmotic stress. The static images suggest a one-way process when the reality involves dynamic feedback loops. Another persistent misconception is that osmosis requires a semipermeable membrane that blocks all solutes. In reality, most biological membranes are selectively permeable. They allow some solutes through while blocking others. The effective osmotic pressure depends on which solutes can cross and which cannot. A solute that crosses freely contributes nothing to the osmotic gradient across that membrane. This is described by the Staverman reflection coefficient, which ranges from zero for freely permeable solutes to one for impermeable ones. I once watched a teaching demo where a professor placed dialysis tubing filled with sucrose solution into water and showed the tubing gaining mass over time. The experiment worked but none of the students understood why glucose in the same setup would produce a very different result. The membrane allowed glucose to diffuse out while water diffused in, creating a complex dynamic that simple mass measurement couldn't capture. Better demonstrations would include real-time measurement of both solute and solvent movement rather than just observing volume change.
Practical Applications Beyond the Lab
Desalination by reverse osmosis is the most widespread industrial application. Pressurizing saline water above its osmotic pressure forces pure water through a semipermeable membrane, leaving salts behind. Modern seawater reverse osmosis membranes operate at pressures around 55 to 80 bar. Energy consumption has dropped significantly over the past decade thanks to improved membrane materials and energy recovery devices. A typical plant now uses about 3 to 4 kilowatt-hours per cubic meter of produced water. Food preservation through salting and sugar curing relies on osmotic principles. High concentrations of salt or sugar create hypertonic environments that draw water out of microbial cells. The lower the water activity, the slower microbial growth becomes. This is why dried foods and cured meats have long shelf lives without refrigeration. The technology is old but the underlying mechanism is still osmosis. Agricultural salinity is a growing problem worldwide. Irrigation water contains dissolved salts that accumulate in soil over time. When soil solution becomes too concentrated, crops experience osmotic stress, effectively suffering from drought despite adequate moisture. Managing this requires leaching salts from the root zone and selecting salt-tolerant crop varieties. I've visited farms where yield losses were attributed to disease when the real cause was osmotic stress from rising soil salinity.
What to Watch For in Experimental Work
If you're setting up osmosis experiments, control temperature precisely. A 5°C variation changes osmotic pressure by roughly 1.7 percent. Use thermostated baths if accuracy matters. Calibrate your instruments before each session. Record ambient conditions. Small deviations compound over time and make reproducibility nearly impossible. When measuring cell volume changes, use phase contrast microscopy rather than brightfield. The contrast makes membrane boundaries much clearer, especially in swollen or shrinking cells. Image analysis software can quantify volume changes with reasonable accuracy if you have a scale bar in every frame. Manual measurements are too error-prone for anything requiring precision. If you're working with plant tissues, be aware that different cell types and tissues have different baseline osmotic potentials. Leaf mesophyll cells differ from root cortex cells, which differ from vascular parenchyma. Sampling strategy matters. Mixing tissue types averages out the variation but obscures real biological differences. I've seen papers report misleading osmotic values because the researchers homogenized multiple tissue types without accounting for the compositional differences.
Membrane integrity testing is essential when using artificial membranes. A tiny leak, even one imperceptible visually, can invalidate results by allowing solutes to bypass the selective barrier. A simple test is to fill the membrane capsule with a dye solution, seal it, and place it in pure water. If the external solution colors over several hours, the membrane has defects and needs replacement.
The Bigger Picture
Osmosis is fundamental to cellular life but it operates within a network of other processes. Ion channels, transporters, osmolyte synthesis, and structural features like cell walls all interact with osmotic forces. Understanding osmosis in isolation gives you a useful tool but understanding it in context gives you insight into how organisms actually function. The difference between knowing the formula and understanding the biology is where real expertise lives. Cells manage osmotic challenges continuously. The kidneys produce up to 180 liters of filtrate daily and reabsorb most of that water through osmotic gradients established by active ion transport. Marine organisms deal with constant water loss in hypertonic seawater through specialized excretory organs and osmolyte accumulation. Freshwater organisms face the opposite problem, constantly gaining water and losing salts, and expend energy to maintain their internal balance. All of these are osmosis-related problems solved by evolution. The process itself is simple in principle. Water moves down its chemical potential gradient across a barrier that discriminates between water and solutes. Complexity arises from the diversity of membranes, solutes, and biological contexts. That's where the actual work happens, in predicting and controlling what happens when those variables shift in ways the textbook doesn't cover.


