Understanding How New Traits Evolve From Ancient Genetic Templates
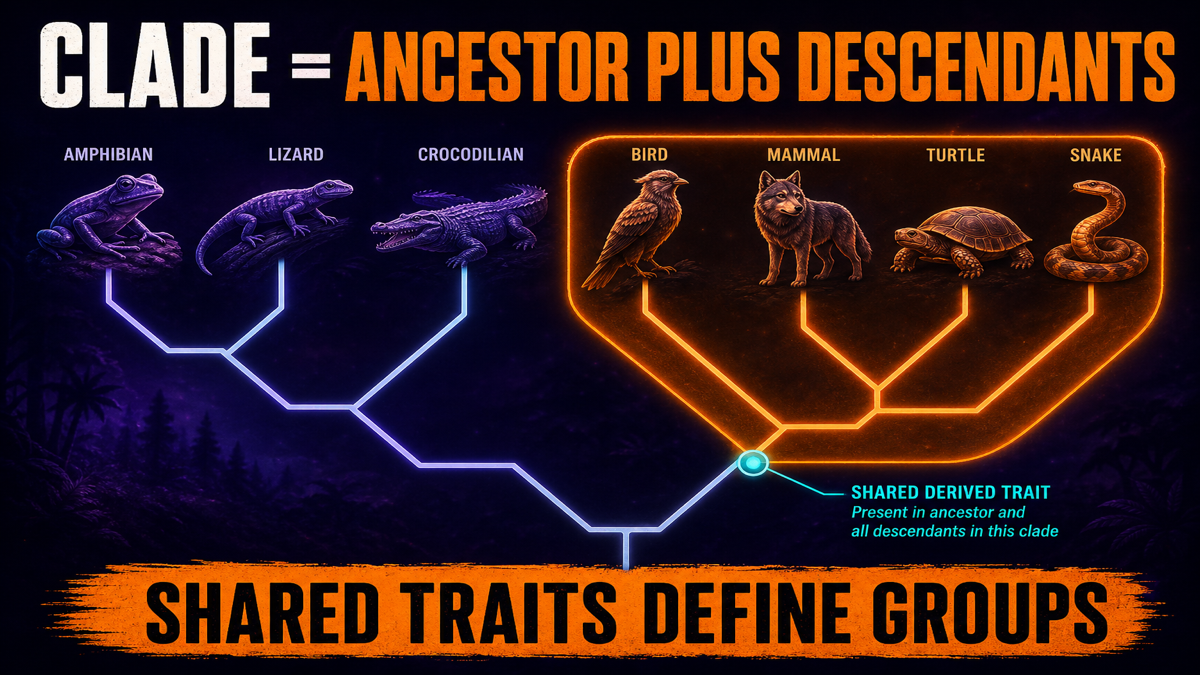
You are probably familiar with the idea that species change over time. What most people do not realize is that this change rarely happens by inventing completely new genetic machinery from scratch. More often, organisms repurpose existing structures and reshape them for entirely different functions. This process creates what biologists call derived traits. These are features that differ from the ancestral condition and typically define specific branches on the tree of life. A derived trait represents an evolutionary modification of a preexisting characteristic. When cladists and systematists trace relationships among organisms, they look specifically for these modifications. The key insight is that a single ancestral blueprint can spawn multiple different forms depending on selective pressure. feathers provide a textbook example. The original function was likely thermoregulation or display, but over millions of years that same basic structure supported powered flight in certain lineages. The underlying anatomical plan remained recognizable even as the functional output changed dramatically. People frequently confuse ancestral and derived traits because the terminology feels counterintuitive. A feature being derived does not mean it appeared recently in absolute time. It only means the trait differs from the ancestral state at a particular node. Sharks have existed longer than mammals, yet sharks retain many ancestral features while mammals exhibit derived conditions. The temporal relationship matters less than the comparative framework.
How Derived Traits Actually Form During Evolution
The mechanism behind trait derivation involves several overlapping processes. Gene duplication provides raw material. When a gene copies itself, one copy can maintain the original function while the other accumulates mutations without immediate fitness cost. Over generations, this second copy may acquire novel expression patterns, new protein interactions, or altered regulatory control. Hox genes demonstrate this principle repeatedly. Modifications in their timing and spatial expression during development produce dramatic morphological changes without requiring new structural components. Regulatory evolution plays an outsized role. Changes to when and where genes express themselves often matter more than changes to the protein-coding sequences themselves. A small shift in developmental timing can relocate a structure, alter its proportions, or modify its functional capacity. This is why two species sharing nearly identical coding genomes can look and behave quite differently. cis-regulatory elements control gene expression without disrupting the core protein product, allowing fine-tuned morphological innovation. I spent considerable time working with comparative genomics data, and one persistent problem I encountered involved distinguishing true homology from convergent similarity. Morphological comparisons alone frequently mislead. I resolved this by integrating developmental gene expression data with phylogenetic context. When a derived trait maps cleanly onto molecular evidence rather than appearing sporadically across unrelated clades, confidence in the interpretation increases substantially. The workaround takes more time initially but prevents expensive revision later.
Why This Matters For Understanding Evolutionary Relationships
Derived traits form the foundation of modern phylogenetic systematics. Wilhelm Hennig introduced cladistics precisely to organize biological diversity using shared derived characteristics rather than overall similarity. Similarity can be deceptive because ancient ancestral traits create false impressions of relationship. Two species may appear closely related simply because both retained primitive features, when in fact each independently derived novel solutions to similar environmental challenges. Modern molecular phylogenetics has refined this approach enormously. DNA sequence data allows researchers to identify synapomorphies with far greater precision than morphology alone. However, the logic remains identical to what Hennig proposed decades ago. Group organisms by shared derived traits. Avoid grouping by shared ancestral traits. This simple rule produces testable, falsifiable hypotheses about evolutionary history. A common pitfall involves treating every difference as informative when it is actually autapomorphic. An autapomorphy is a derived trait unique to a single species. It provides no information about relationships with other organisms. When building phylogenetic trees, these unique modifications must be recognized and excluded from grouping decisions. Beginners often include autapomorphies as evidence for relationships, which inflates branch support artificially.
Get the Full Details

Real-World Examples Of Ancestral Repurposing
The vertebrate limb illustrates how effectively ancestral blueprints adapt. The basic pentadactyl pattern appears in amphibians, reptiles, birds, and mammals. Despite dramatic functional differences between a bat wing, a whale flipper, and a human hand, the underlying skeletal arrangement remains strikingly consistent. Modifications occurred through changes in bone proportions, fusion events, and loss of certain elements. The developmental toolkit controlling limb formation is ancient, but the outputs vary enormously across lineages. Mammalian ear bones represent another compelling case. Three bones once part of the jaw joint became incorporated into the middle ear of mammals. This transition required precise coordination between skeletal reduction and auditory enhancement. Fossil intermediates document this change progressively. The same bones serving chewing in early synapsids gradually shifted toward sound transmission in mammalian descendants. Functional repurposing did not require new genetic material. It required rewiring existing connections. Bird teeth provide a useful cautionary example. Modern birds lack teeth, but their ancestors possessed them. Several research groups attempted to reactivate tooth development in chicken embryos using retroviral vectors. The experiments produced tooth-like structures with reasonable fidelity. This demonstrates that the genetic potential for teeth persists beneath the surface even when the trait appears lost. Ancestral blueprints remain available for evolutionary exploitation given the right selective conditions.
Potential Limitations And Misinterpretations
Not every visible difference qualifies as a derived trait worth evolutionary attention. Some modifications arise from genetic drift rather than selection. Neutral changes accumulate continuously and can create apparent divergence that has no adaptive significance. Distinguishing neutral from selected changes requires population-level data and statistical testing. Morphology alone cannot make this distinction reliably. Phenotypic plasticity complicates trait classification as well. Organisms sometimes alter their appearance in response to environmental conditions without any genetic change. If researchers record plastic phenotypes as fixed species characteristics, phylogenetic analyses become unreliable. Common garden experiments and reciprocal transplants help separate environmentally induced variation from heritable derived traits. These controls add time and resources to studies but prevent systematic error. Molecular convergence represents another concern. Similar DNA changes can arise independently in unrelated lineages facing comparable selective pressures. This creates false synapomorphies that mislead phylogenetic reconstruction. Examining multiple independent loci and using model-based methods that account for convergent substitution rates reduces this risk. No single gene tells the whole story about evolutionary relationships.
Practical Approaches To Identifying Derived Traits
Constructing a character matrix requires careful consideration of trait scoring. Each character should represent a heritable feature with definable states. Continuous traits sometimes resist clean categorization. Breaking them into discrete intervals introduces arbitrary boundaries but enables numerical analysis. Researchers increasingly apply continuous character models to avoid this discretization problem entirely. Fossil evidence improves character polarization significantly. Determining whether a trait is ancestral or derived requires outgroup comparison. The outgroup should resemble the hypothesized ancestral condition without sharing the derived modification. Selecting appropriate outgroups matters. Too distant a relative may share so few characteristics that polarization becomes impossible. Too close a relative may itself possess derived traits that obscure the pattern. I have found that documenting character transformations directly alongside phylogenetic trees provides the clearest communication of results. Animated reconstructions showing trait changes across branches help readers grasp complex evolutionary sequences more effectively than static tables. This approach requires more effort during manuscript preparation but pays dividends through increased citation and clearer scientific messaging.

Why The Concept Continues To Shape Biological Research
The derived trait framework connects disparate subdisciplines within evolutionary biology. Paleontologists use it to interpret fossil sequences. Developmental biologists examine how modifications arise during ontogeny. Ecologists investigate the selective pressures driving trait diversification. Conservation biologists apply the logic to identify evolutionarily significant units within endangered populations. Future research directions increasingly emphasize the integration of genomics, development, and ecology. The field moves beyond cataloguing derived traits toward understanding the mechanistic basis of trait evolution. Which genes control morphological innovation. How regulatory networks rewire during adaptation. What ecological opportunities trigger rapid trait diversification. These questions build on the traditional derived trait framework while extending it into new methodological territory. Evo-devo research has revealed that deeply conserved developmental pathways repeatedly generate novel forms through modification of timing, location, and intensity. The genetic mechanisms underlying innovation are often simpler than previously assumed. Small changes to regulatory sequences produce large morphological effects. This parsimony suggests that evolutionary transformation may be more accessible than classical population genetics models alone would predict.