Cellular Respiration Isn't As Clean As Your Textbook Makes It Sound
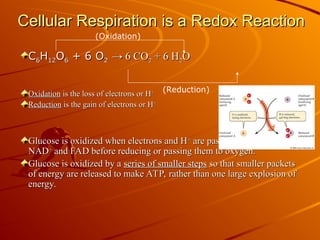
We all learned the equation in high school biology: glucose plus oxygen yields carbon dioxide, water, and ATP. Six CO2, six H2O, roughly thirty to thirty-two ATP molecules depending on how efficient your electron transport chain is being that day. It's elegant. It's simple. It's also incomplete. The reality is messier. Every cell in your body is running a continuous combustion engine that produces not just the clean waste products listed above, but a whole cascade of toxic intermediates and byproducts that accumulate over time. I spent a good chunk of my career studying mitochondrial dysfunction and reactive oxygen species, and the thing that always surprised me was how casually most people dismiss the waste.
The Dark Side Of Cellular Respiration The Good The Bad And The Toxic Waste Products We Produce
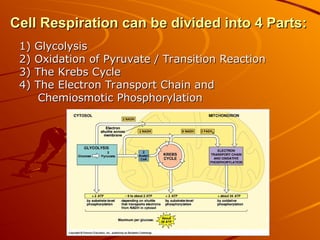
Let's start with what actually gets produced beyond ATP and water. The electron transport chain runs four protein complexes embedded in the inner mitochondrial membrane. Complexes one through four pass electrons from NADH and FADH2 to oxygen, which sits at the very end as the final electron acceptor. Oxygen gets reduced to water in the process. That part is clean. Except it isn't entirely. About one to two percent of the oxygen that enters the chain leaks out before it gets fully reduced, picking up a single electron instead of two. This creates superoxide anion, O2 minus. It sounds minor but it's the root of most downstream problems. Superoxide gets converted by superoxide dismutase into hydrogen peroxide, which is less reactive but still damaging, and then into water by catalase or glutathione peroxidase. Under normal conditions this scavenging system works fine. Under stress conditions, or as we age, it falls behind. Here's what most introductory courses don't tell you: the reactive oxygen species produced during respiration aren't just accidental byproducts. They're signaling molecules. Low levels of H2O2 trigger adaptive responses like upregulating antioxidant defenses and promoting mitochondrial biogenesis through pathways involving Nrf2 and PGC-1alpha. The problem emerges when production outpaces detoxification. That's when you get lipid peroxidation of membrane phospholipids, oxidation of protein thiols, and DNA damage including the notorious 8-oxoguanine lesion in mitochondrial DNA.
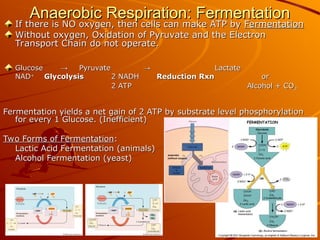
I ran into this directly when working with cell culture models of exercise adaptation. We were trying to measure whether acute exercise increased mitochondrial efficiency or just increased ROS production. The standard assays for ATP production and oxygen consumption rate gave conflicting results. Some samples showed higher coupling efficiency while simultaneously showing higher H2O2 emission. It turned out the cells were compensating by upregulating antioxidant enzymes, which temporarily masked the damage but didn't eliminate the source. The workaround was using MitoSOX for superoxide-specific detection combined with Seahorse analysis of spare respiratory capacity. The combination gave us data that neither assay could provide alone. Standard NADH/FADs missed the whole picture because they don't distinguish between coupled and uncoupled respiration. Beyond ROS, there are other waste products worth tracking. When oxygen availability drops even slightly, cells shift toward partial reduction of pyruvate to lactate. Lactate itself isn't toxic, but the accompanying proton accumulation drops intracellular pH and disrupts enzyme function. This is why intense exercise causes the burning sensation, and why conditions like ischemia can be rapidly destructive. The brain is especially vulnerable because neurons rely almost exclusively on aerobic respiration and have minimal glycogen stores. Another underappreciated product is methylglyoxal, a reactive dicarbonyl compound formed as a side reaction during glycolysis. It's produced continuously at low rates but spikes when glycolytic flux is high, which happens during high-carbohydrate states or insulin resistance. Methylglyoxal modifies proteins through advanced glycation end-products, and the body detoxifies it primarily through the glyoxalase system using glutathione. When that system gets overwhelmed, you see increased AGE accumulation in tissues, which contributes to vascular stiffness and neurodegeneration independent of blood glucose levels.
Get the Full Details

There's also the issue of mitochondrial DNA damage being particularly problematic. Unlike nuclear DNA, mtDNA lacks histone protection and sits right next to the electron transport chain where ROS is generated. The repair mechanisms are limited, mostly base excision repair through OGG1 and APE1. Mitochondria can't afford double-strand breaks the way nuclear DNA can because they lack robust non-homologous end joining. This means mutations accumulate with age, leading to respiratory chain deficiencies in individual cells. When enough mitochondria in a cell become dysfunctional, the cell undergoes apoptosis or contributes to senescent phenotype secretion. The ketone bodies often get labeled as alternative fuel sources, which they are, but they're also waste management products. When carbohydrate availability is low and acetyl-CoA from fatty acid oxidation exceeds what the TCA cycle can handle, the liver shunts excess acetoacetyl-CoA into ketone bodies, particularly beta-hydroxybutyrate and acetoacetate. These cross the blood-brain barrier and serve as fuel for neurons during fasting or ketogenic states. The catch is that ketone production itself increases mitochondrial ROS initially, and prolonged ketosis without adequate electrolyte balance can lead to ketoacidosis, especially in type one diabetes where insulin deficiency prevents proper ketone utilization. If you're dealing with this practically, whether in research or clinical contexts, here's what I've found useful. First, don't rely on a single metric. ATP levels, oxygen consumption, ROS production, and membrane potential all tell different parts of the story. Measuring just one gives you a distorted view. Second, pay attention to the redox state of the matrix. The NADH/NAD+ ratio directly affects dehydrogenase activity and thus TCA cycle flux. When this ratio gets too high, the cycle backs up and electrons pile up in the chain, increasing ROS leakage dramatically. Third, consider the permeability transition pore. Under calcium overload or oxidative stress, this pore opens permanently and collapses membrane potential, causing mitochondrial swelling and release of cytochrome c. It's essentially the point of no return for that organelle.
The bottom line is that cellular respiration is efficient but not clean. The same process that generates most of your ATP also produces the molecular damage associated with aging and many diseases. The body has evolved countermeasures, and they work well most of the time. But they're not perfect, and understanding what gets produced, when, and how the body handles it gives you a much more complete picture than the simplified equation ever will.