Understanding the Carbohydrate Code and the Carbs Monomer
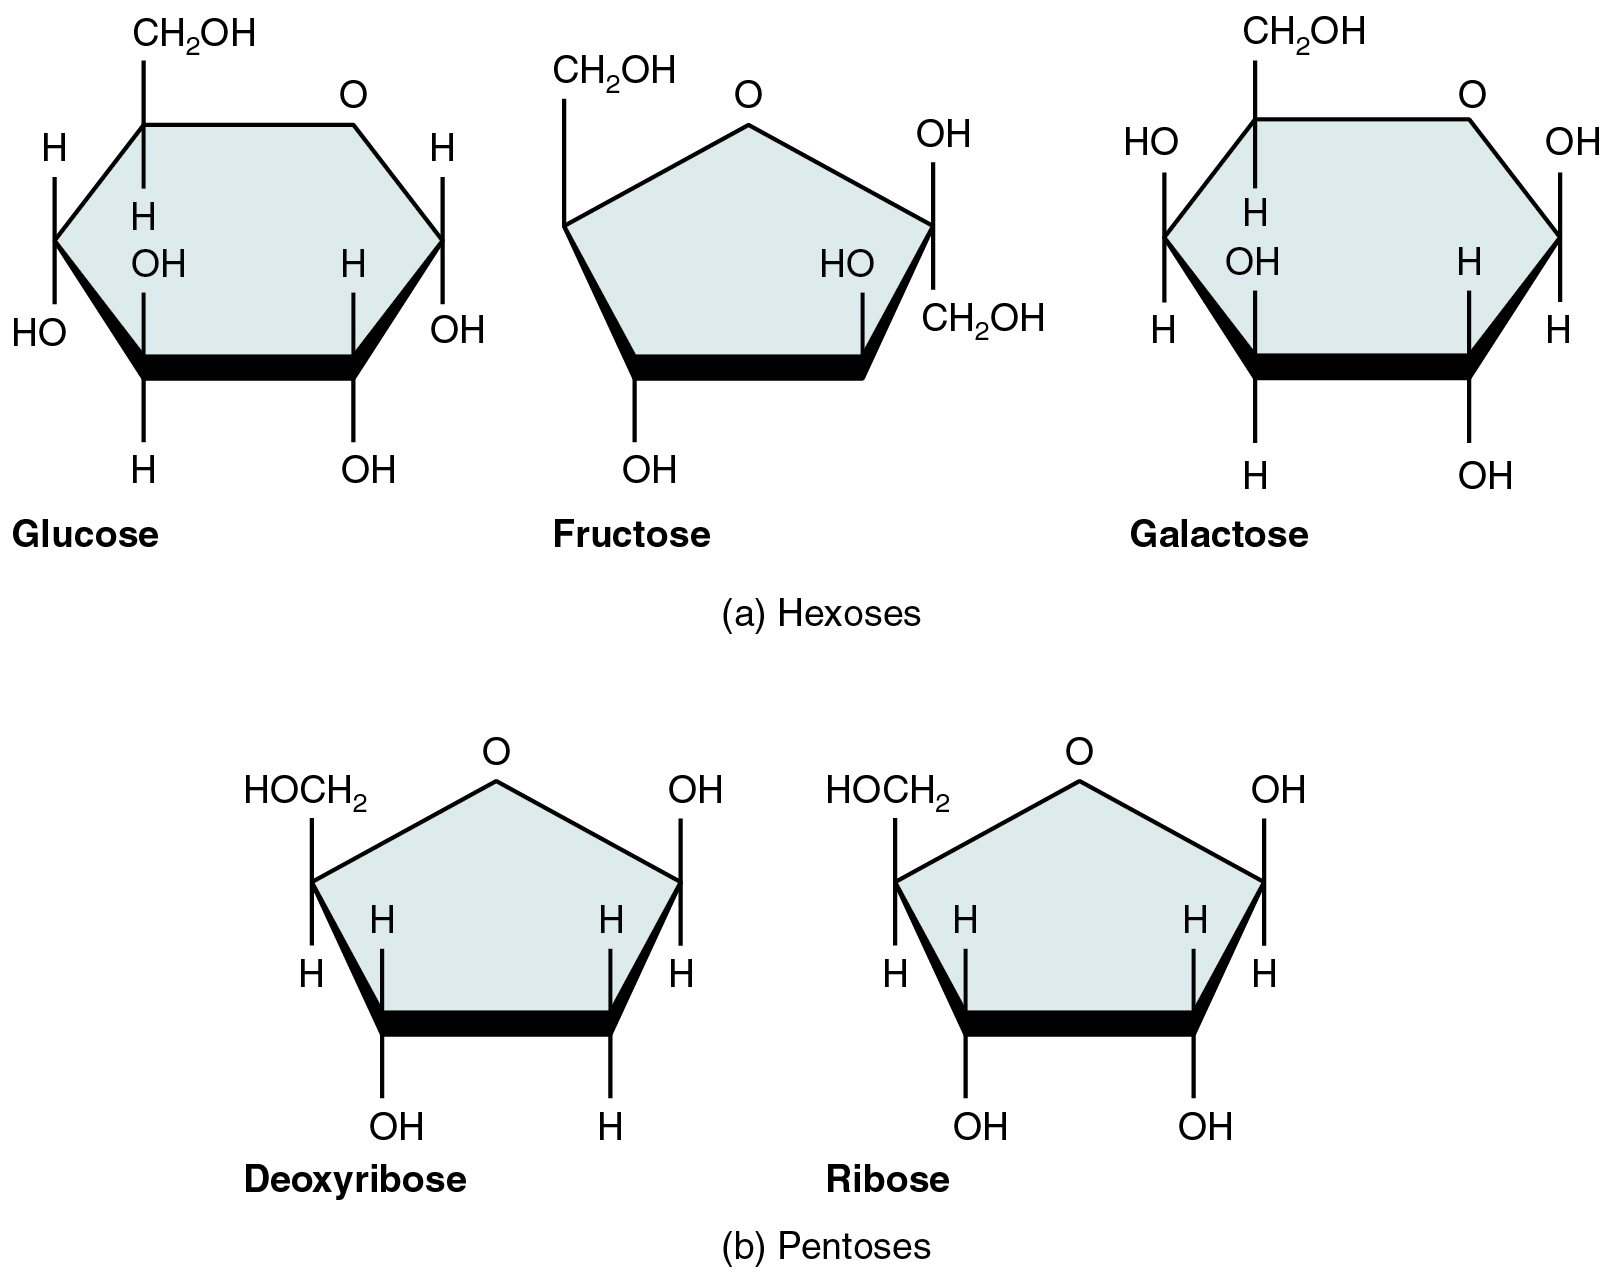
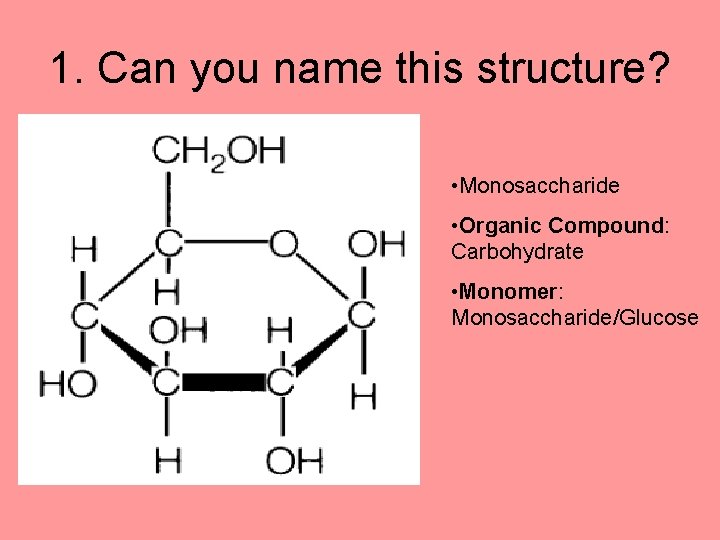
When you look at how living systems store and use energy, the monomer units of carbohydrates are where the real story starts. This is what I mean by The Carbohydrate Code How The Carbs Monomer Dictates Energy Structure And Life Itself — it is not a formal scientific term, but it describes something very real that happens at the molecular level. The monomer of carbohydrates is a simple sugar, most commonly glucose, fructose, or galactose. These are monosaccharides with the general formula CnH2nOn. A single glucose molecule has six carbon atoms, twelve hydrogen atoms, and six oxygen atoms arranged in a specific three-dimensional pattern. That arrangement is not arbitrary. It determines how the molecule folds, how enzymes recognize it, and whether it gets broken down for immediate energy or packaged into storage structures. I spent years working in a lab studying polysaccharide synthesis and degradation pathways. The thing nobody tells you upfront is that the difference between starch and cellulose is literally one bond angle. Both are made of glucose. Starch uses alpha-1,4-glycosidic linkages and forms helical structures that enzymes can quickly access. Cellulose uses beta-1,4-glycosidic linkages and stacks into rigid linear sheets held together by hydrogen bonding. Humans have the enzymes to digest starch. We cannot digest cellulose at all. The same monomer. Entirely different biological outcomes.
How the Monomer Structure Dictates Energy Architecture
The way a carbohydrate monomer is configured controls everything downstream. Glycogen in animals, for instance, is a highly branched polymer of glucose with alpha-1,6-linkages appearing roughly every ten to fourteen residues. That branching pattern is not decorative. It creates thousands of accessible chain ends where glycogen phosphorylase can simultaneously cleave glucose units. More branches mean faster mobilization when your blood sugar drops. I once ran into a problem where we were trying to quantify glycogen breakdown rates in liver tissue samples and the values kept coming back inconsistent. The issue was that glycogen structure itself varies depending on the metabolic state of the animal. Fasted animals had fewer branches and longer outer chains compared to fed animals, and our standard assay conditions favored only the rapidly accessible outer chains. We were effectively measuring only a fraction of the total glycogen pool. The workaround was switching to a dual-enzyme approach — using both glycogen phosphorylase and debranching enzyme together under extended incubation times of about 45 minutes instead of the usual 10. That brought the measured values into line with what we expected based on tissue weight and known glycogen concentrations.
Metabolic Recognition and Enzyme Specificity
Every enzyme that processes carbohydrates has an active site shaped to fit a specific monomer configuration. Hexokinase phosphorylates glucose at the sixth carbon. Glucokinase does the same but with a much higher Km, meaning it only becomes active when glucose concentrations are elevated after a meal. These differences are not academic details. They determine which tissues respond first to a spike in blood sugar and which wait for a sustained signal. The pentose phosphate pathway is another place where monomer structure becomes critical. Glucose-6-phosphate enters this pathway instead of glycolysis, and the first committed step produces ribulose-5-phosphate, a five-carbon sugar. That ribose backbone gets used to build ATP, NADPH, and nucleotide precursors. If your cells need to divide rapidly, that pathway ramps up. If they need reducing power for detoxification reactions, it shifts direction. The same starting molecule. Different metabolic destinations based entirely on cellular demand and allosteric regulation.
Get the Full Details
Common Misunderstandings About Carbohydrate Structure
There is a persistent idea that simple carbohydrates are inherently bad and complex carbohydrates are inherently good. That framing is too blunt to be useful. A monosaccharide like glucose is chemically simple, but the body treats it the same way regardless of whether it comes from a piece of fruit or a processed food. The difference lies in the matrix — fiber, water content, protein, and fat all modulate absorption rate and the resulting metabolic response. Another misconception is that all sugars are equal. Fructose and glucose share the same molecular formula, C6H12O6, but their structures differ. Fructose has a ketone group while glucose has an aldehyde group. That small difference means fructose is metabolized almost entirely in the liver, bypassing the insulin-dependent glucose uptake mechanism. At moderate intakes this is fine. At high levels, particularly from isolated fructose rather than whole fruit, it contributes to de novo lipogenesis and can overwhelm hepatic processing capacity within hours.
The Role of Glycosidic Bonds in Structural Polysaccharides
Glycogen, starch, and cellulose are all polymers of glucose, but the glycosidic bond geometry determines whether the result is an energy reserve, a structural component, or something that passes through the digestive tract unchanged. Hemicellulose and pectin add further complexity. These are heteropolysaccharides made from multiple types of monosaccharides — xylose, arabinose, galactose, and uronic acids — linked in patterns that vary by plant species and tissue type. When you study carbohydrate structure in practice, you quickly learn that the same monomer can participate in very different linkage positions. Galactose in lactose uses a beta-1,4 linkage to glucose. In agarose, galactose derivatives form the repeating disaccharide unit through alternating alpha-1,3 and beta-1,4 bonds, creating a gel matrix that bacteria and some eukaryotes use as a structural scaffold. One monomer, multiple biological roles depending on how it is connected.
Practical Considerations for Working with Carbohydrate Systems
If you are working in a lab setting or trying to understand metabolic data, here is what actually matters. First, always confirm the anomeric configuration of the glycosidic bonds you are studying. Alpha and beta linkages respond differently to acid hydrolysis and enzymatic cleavage. Second, be aware that glycogen and starch granules are semi-crystalline. The outer amorphous regions degrade faster than the inner crystalline zones, which means kinetic measurements can be misleading if you do not account for granule accessibility. I learned this the hard way when comparing in vitro digestion models across different starch sources. A standard amylopectin-rich corn starch degraded to about 85 percent within thirty minutes under simulated intestinal conditions, while a high-amylose variant reached only 30 percent in the same timeframe despite identical enzyme concentrations. The difference was not the glucose monomer itself but the packing density created by linear amylose chains forming helical inclusion complexes. This matters enormously if you are building a model to predict glycemic response or designing a drug delivery system based on carbohydrate matrices.

Where This Framework Falls Short
The carbohydrate monomer-centric view does not explain everything. Non-carbohydrate molecules heavily influence how carbohydrates are processed. Dietary fiber affects glucose absorption through physical entrapment and fermentation into short-chain fatty acids. Protein and fat slow gastric emptying, which changes the temporal profile of monomer appearance in the bloodstream. Hormonal signals like insulin and glucagon override direct monomer concentration in many tissues. Focusing exclusively on the monomer structure gives you the foundation, but the actual biology operates at a systems level that requires additional variables to model accurately. If you need a more complete picture, you have to incorporate transport kinetics, hormonal regulation, and tissue-specific enzyme expression patterns into whatever framework you are using. The monomer is the starting point. It is not the whole story.
Bottom Line
The arrangement of atoms in a single glucose molecule determines whether it becomes quick energy, stored fuel, a structural polymer, or an undigested fiber passing through your system. The glycosidic bond type, the branching pattern, and the three-dimensional conformation collectively encode far more information than the monomer formula alone suggests. Understanding this is useful whether you are interpreting metabolic data, designing experiments, or just trying to make sense of why the same sugar behaves differently depending on where it comes from.