Understanding the Biosphere Beyond the Textbook Definition
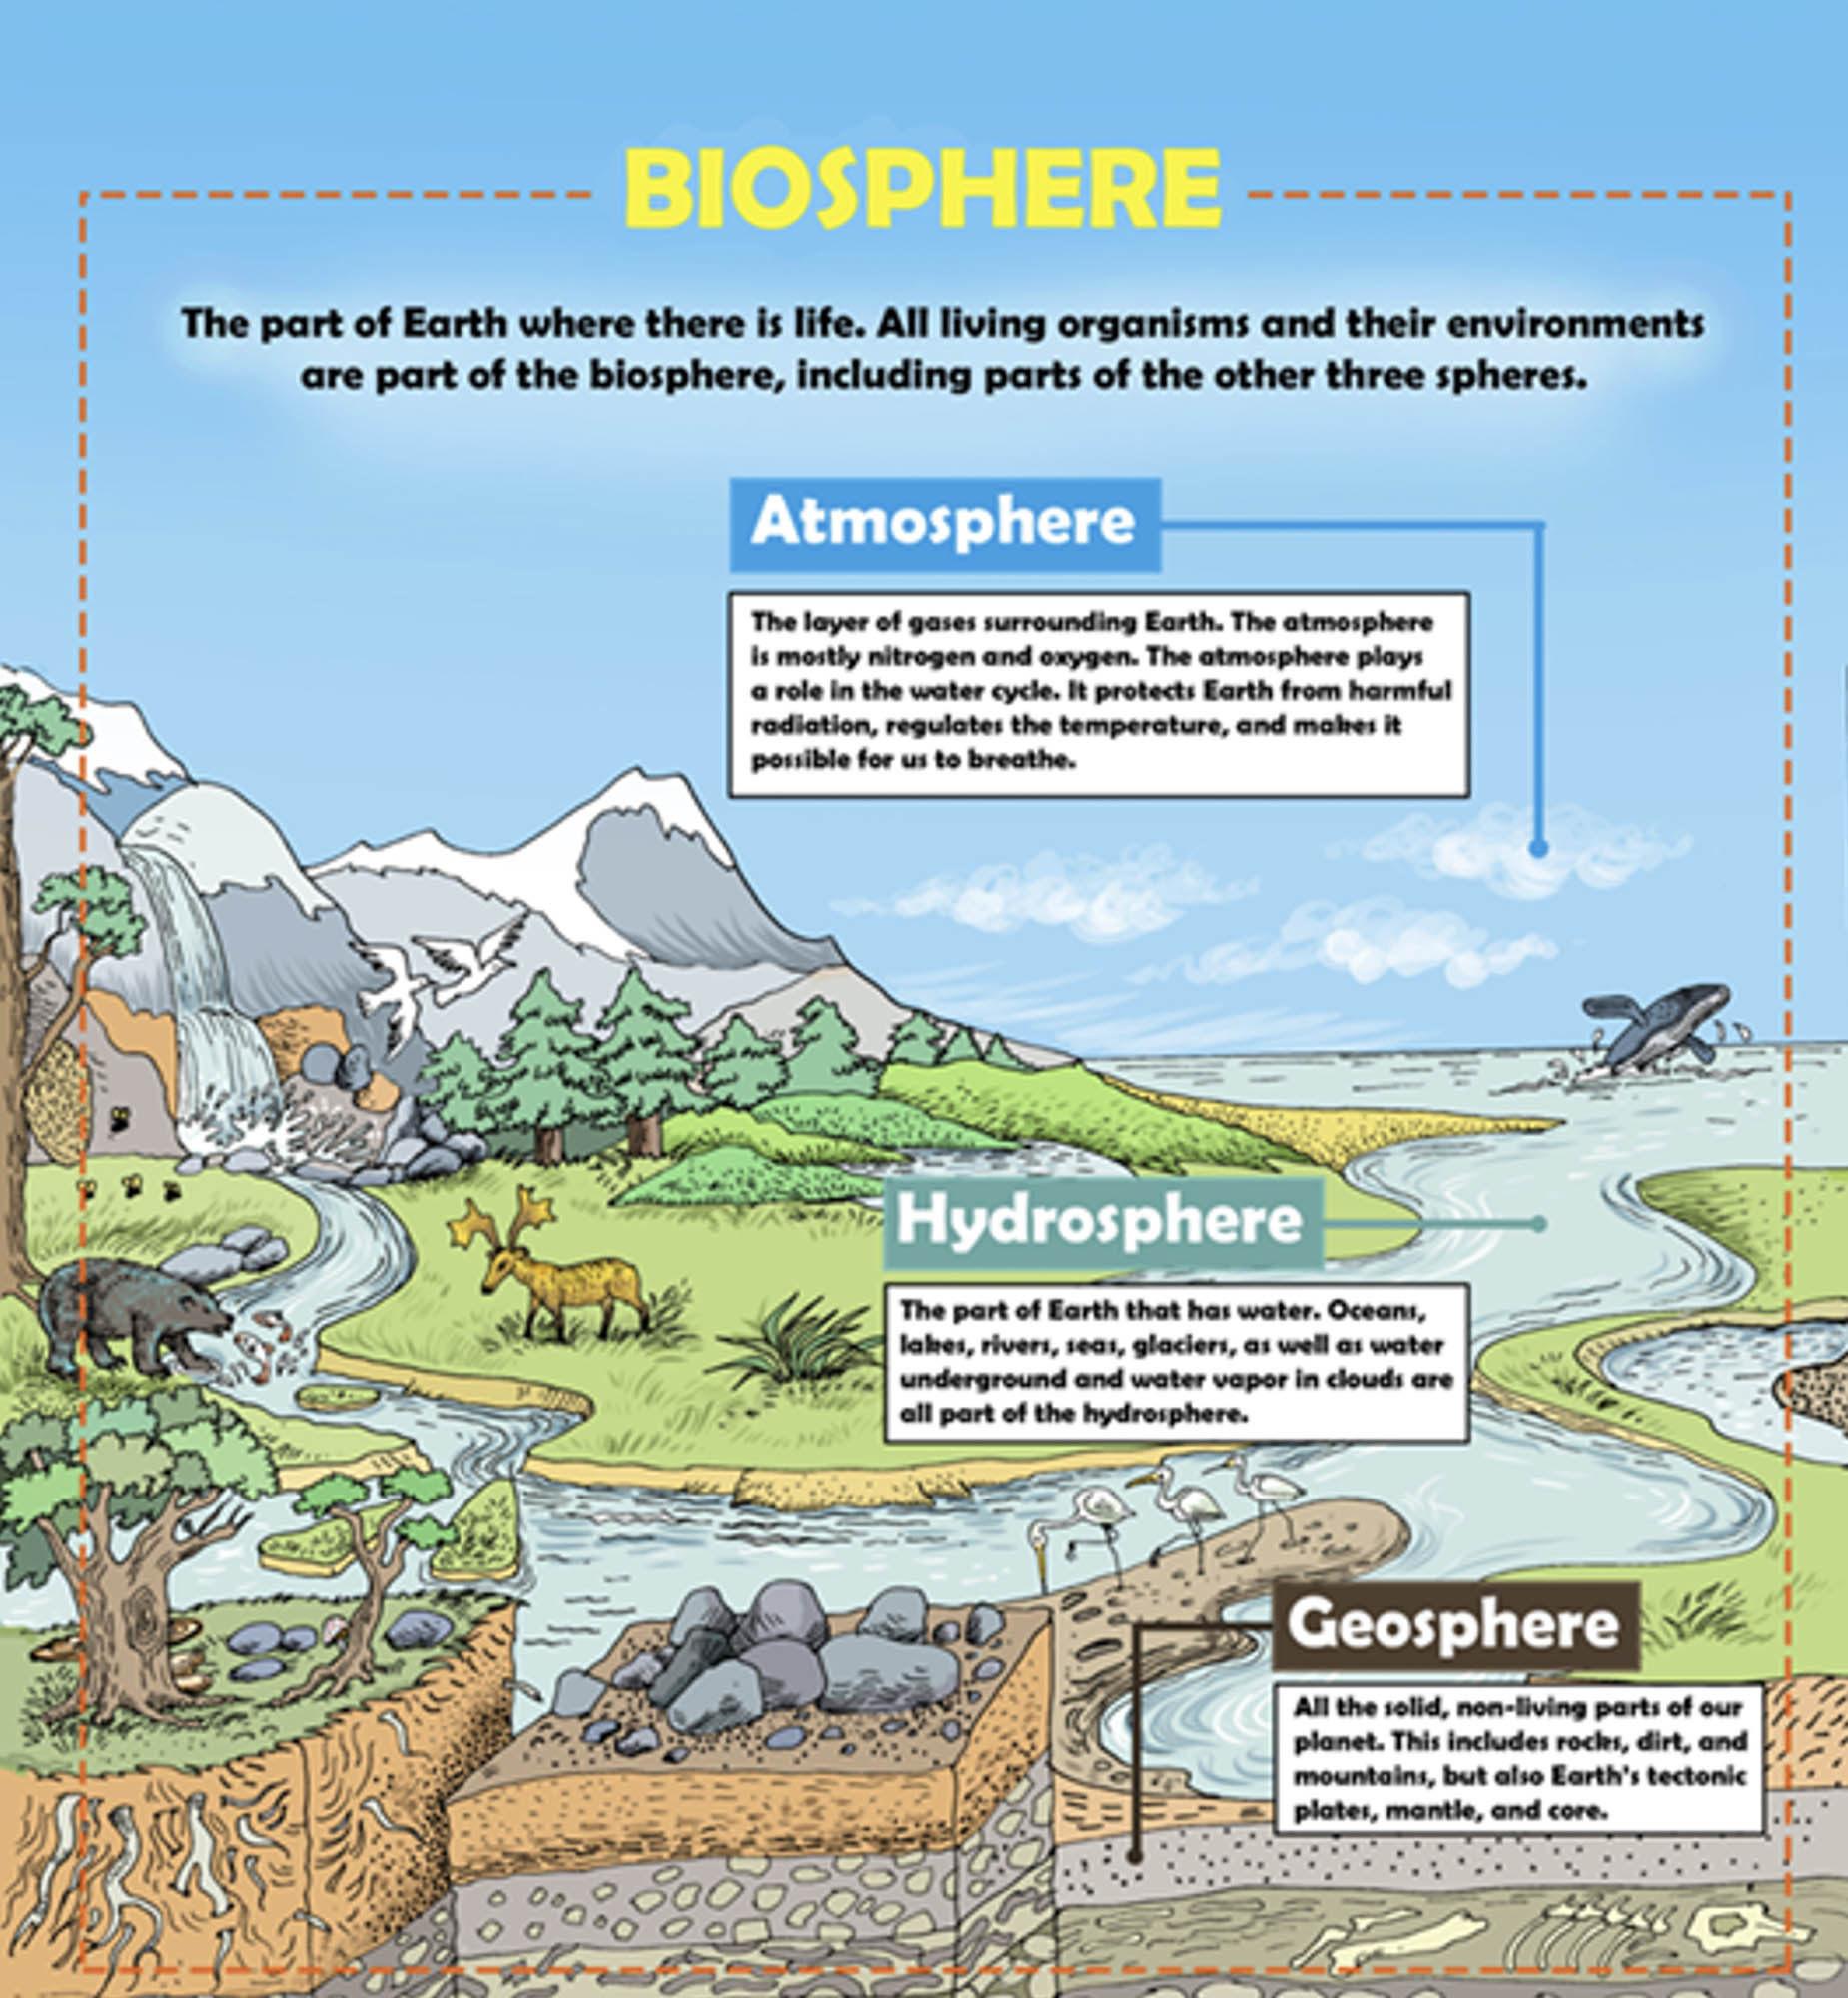
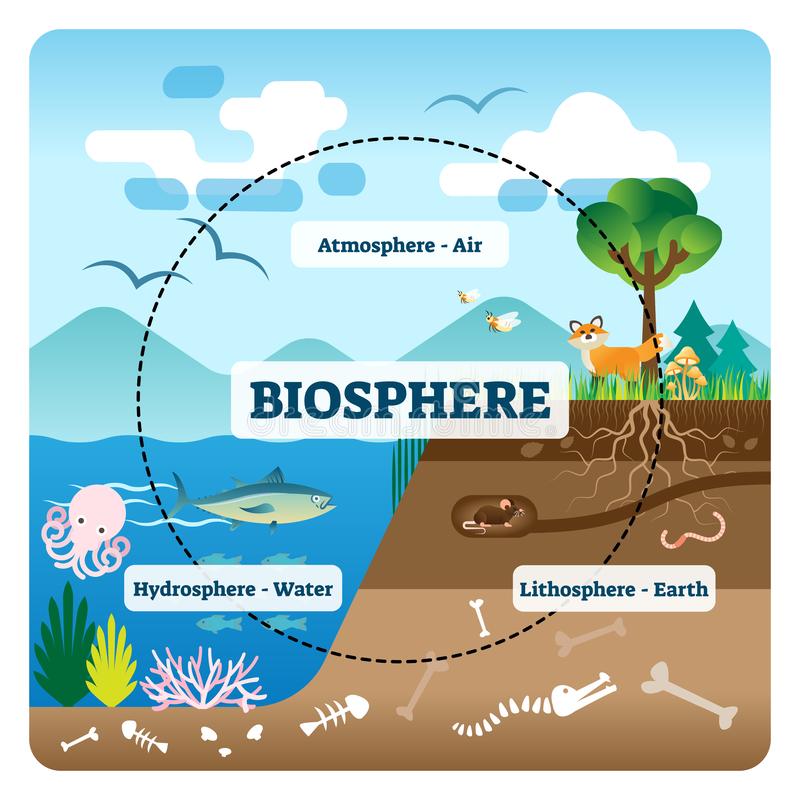
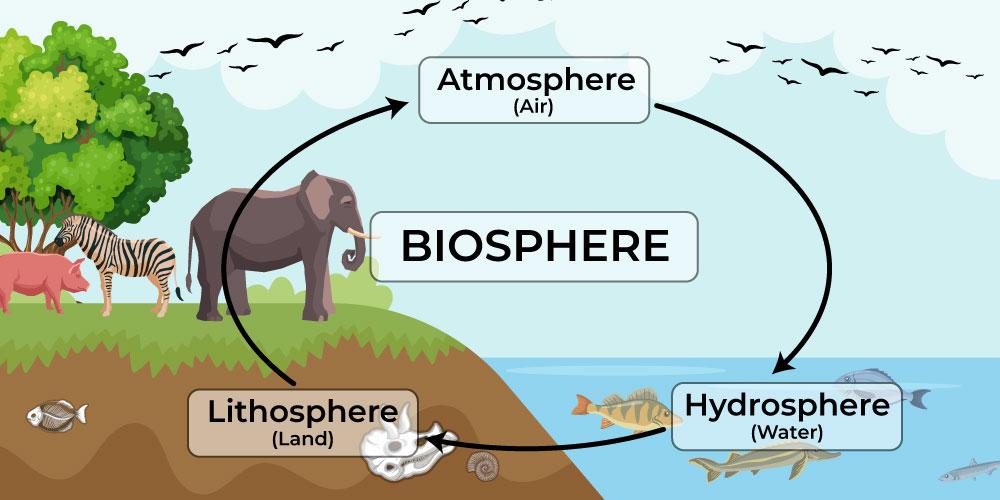
Most people think of the biosphere as the thin strip of life on Earth's surface. They picture soil, trees, oceans, and the creatures in them. That's not wrong, but it's incomplete. The biosphere extends from about 10 kilometers above sea level in the atmosphere down to roughly 11 kilometers below the ocean surface in the hadal zones. It also exists miles beneath the crust in subsurface rock formations where microbes metabolize minerals without any sunlight at all. This vertical range matters more than textbooks usually admit. When you actually study how these zones interact, things get messy quickly. The boundary between the lithosphere, hydrosphere, atmosphere, and the living component isn't clean. It's fuzzy and constantly shifting. You can't map it precisely because biological activity modifies its own boundaries in real time.The Boundless Web Of Life Understanding What Is A Biosphere
A biosphere functions through continuous cycling of matter and energy transfer between organisms and their physical environment. Carbon moves from atmospheric CO into plant tissue through photosynthesis, then into herbivores, then into predators, then back into the atmosphere through respiration or decomposition. Nitrogen follows a similarly complex route involving fixation, nitrification, and denitrification, each step carried out by specific microbial communities. Phosphorus cycles more slowly because it lacks a significant atmospheric component. It moves primarily through weathering of rocks, uptake by organisms, sedimentation, and eventual geological uplift. Energy flows through this system in one direction. It enters as solar radiation, gets converted to chemical energy by primary producers, and dissipates as heat at every trophic level. Roughly 10 percent of the energy at one trophic level transfers to the next. The rest is lost as metabolic heat. This 10 percent rule is why food chains rarely exceed five or six links and why top predators always exist in lower densities than their prey.
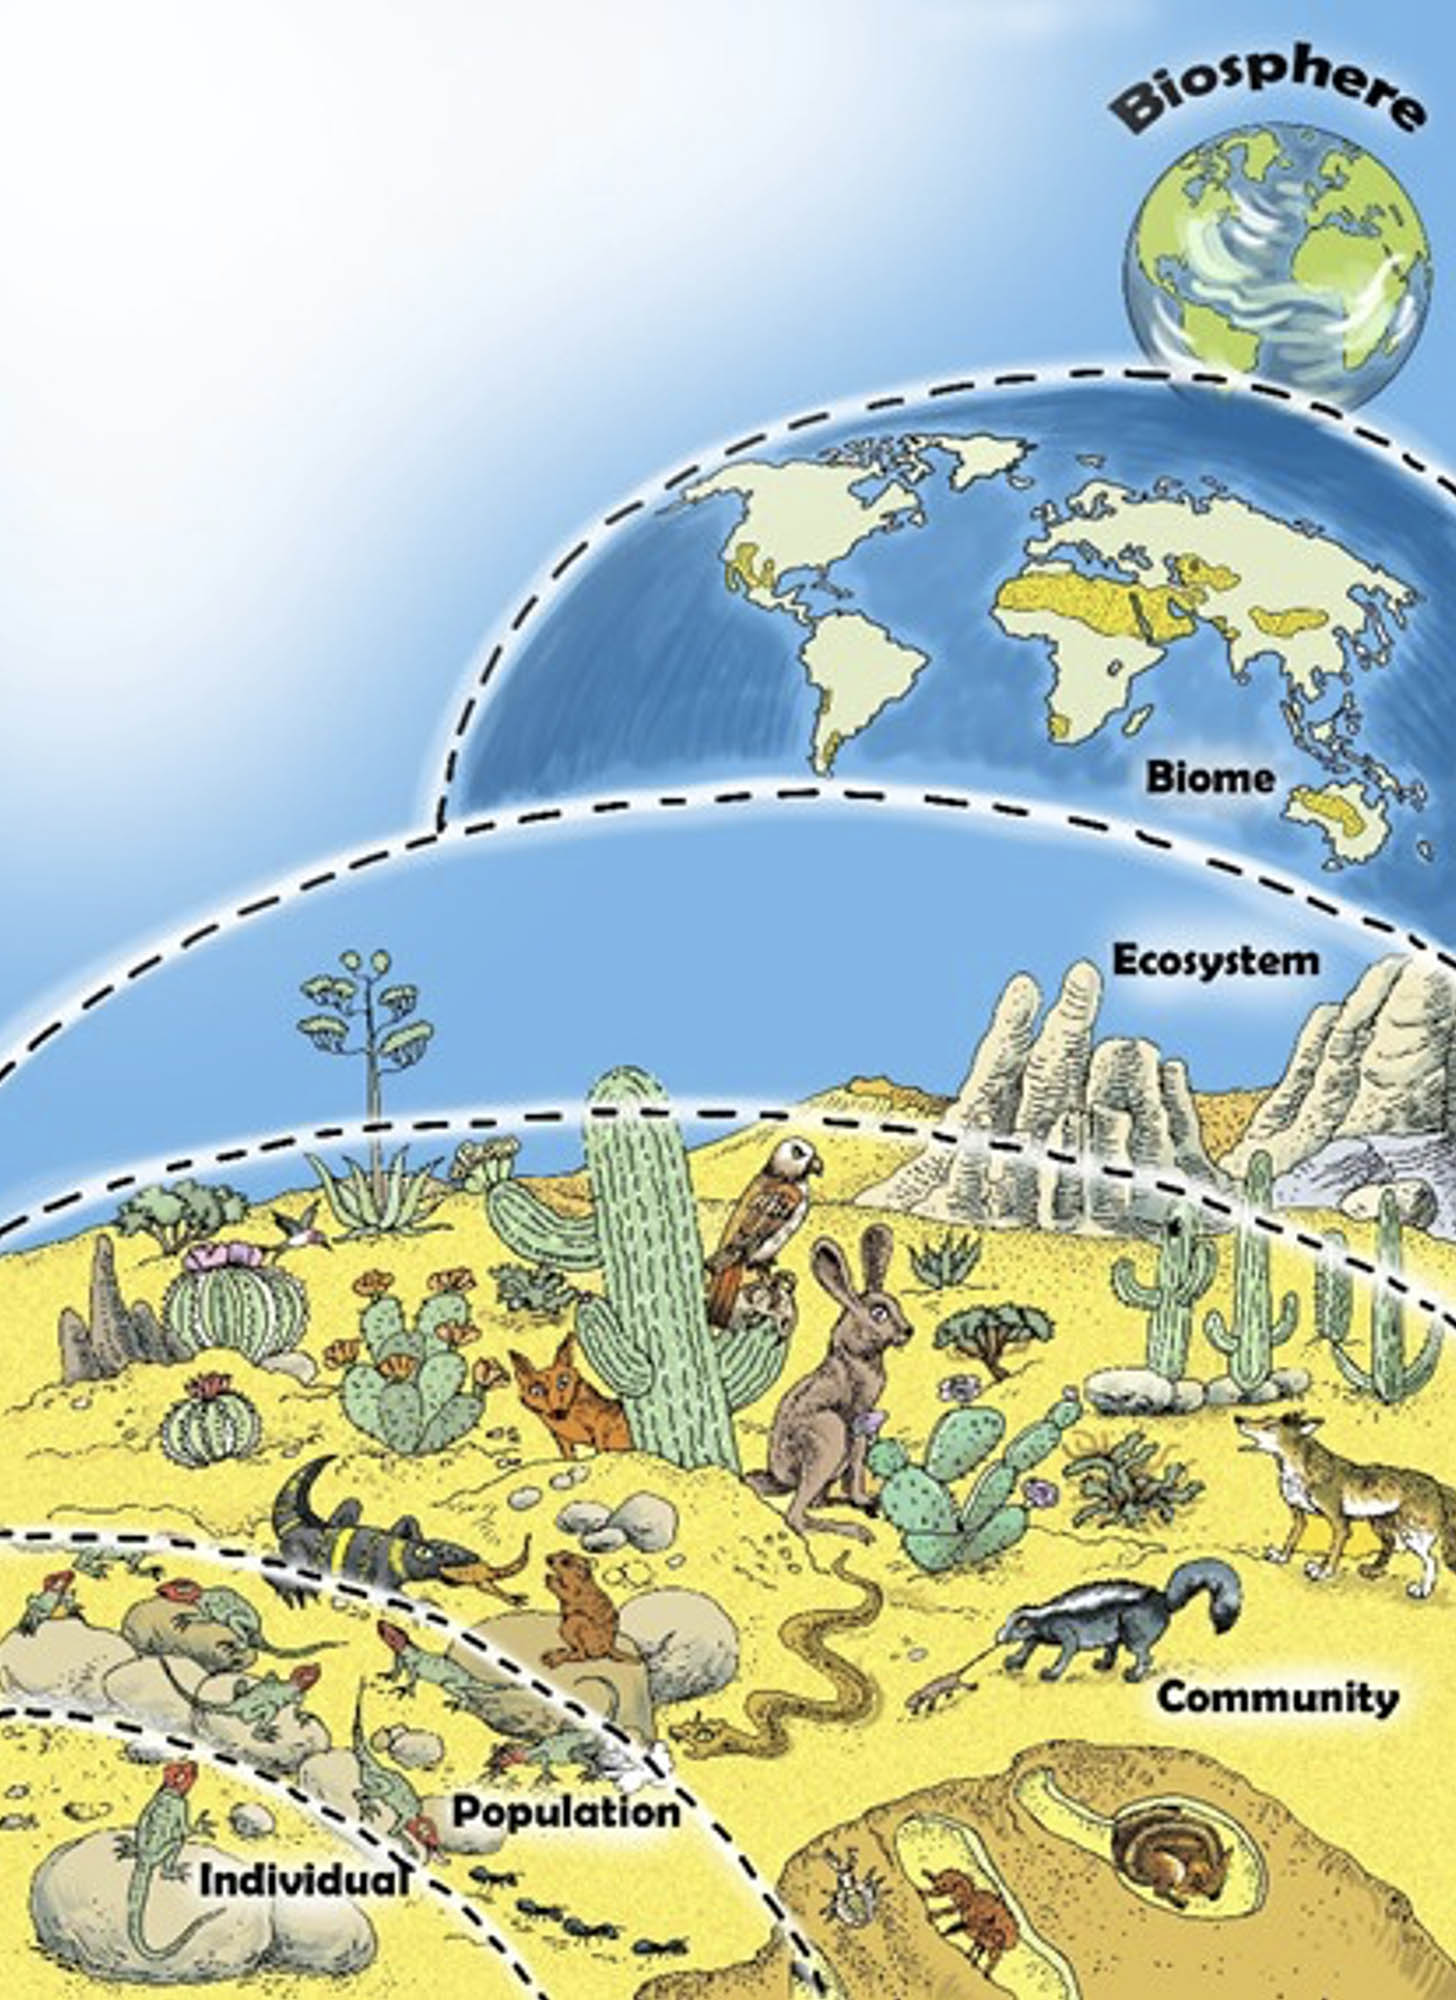
I ran into a concrete problem last year modeling nutrient fluxes in a high-altitude alpine ecosystem. Standard models treated the permafrost layer as a static boundary, but my field data showed that thaw pockets were releasing ancient organic carbon at rates far higher than the model predicted. The discrepancy came from a single oversight: the model didn't account for cryoconite holes forming on retreating glacier surfaces. These are dark, microbial-rich pools that absorb significantly more solar radiation than surrounding ice, accelerating localized melting and creating micro-environments where previously frozen carbon becomes biologically active again. I spent three weeks recalibrating the model parameters, adding permafrost vulnerability as a dynamic variable rather than a fixed threshold. The revised output shifted the estimated carbon release by nearly 40 percent over a twenty-year projection window. That's the kind of gap you only find when you're actually working with the system instead of reading about it. Most beginners treat biomes as static categories. They learn the list: tropical rainforest, temperate deciduous forest, taiga, tundra, desert, grassland, coral reef, freshwater. Then they assume these zones stay put. In practice, biome boundaries shift continuously in response to temperature, precipitation, fire regimes, and species migrations. The treeline moves. Desert margins expand and contract. Permafrost degradation is pushing tundra ecosystems toward shrubland dominance across large sections of the Arctic. These aren't gradual changes you'd notice in a human lifetime if you just glance at a map once a decade. They're measurable and accelerating in many regions. Another thing that trips people up is the assumption that biodiversity equals stability. Higher species richness generally improves ecosystem resilience, but the relationship isn't linear or guaranteed. Some highly diverse systems collapse under relatively minor perturbations if the critical structural species are removed. A coral reef with thirty fish species can disappear in months if the grazing parrotfish population crashes and algae overgrows the substrate. The diversity was there. The functional redundancy wasn't. Losing one keystone species can trigger cascading failure across multiple trophic levels regardless of how many other species remain. There's no single tool that captures the full complexity of a biosphere. Satellite remote sensing gives you broad coverage of vegetation indices and land surface temperature but misses everything underground and most of the microbial dimension. Environmental DNA sampling reveals organism presence without showing abundance or behavior. Eddy covariance towers measure carbon and water flux at a point, but extrapolating those measurements across landscapes introduces significant uncertainty. Isotopic tracing works well for specific pathways but gets expensive and labor-intensive quickly. The most reliable approach combines multiple methods and accepts that each has blind spots. Biogeochemical models like the ones used by the IPCC attempt to integrate all these data streams, but they're constrained by resolution and parameter uncertainty. They tend to smooth over the very heterogeneity that makes real ecosystems function the way they do. Local-scale processes get lost in global averages. This doesn't make the models useless. It means you need to understand what they're actually capable of representing before you trust their outputs for anything specific. The biosphere doesn't have clean edges. It has gradients and overlap zones where multiple systems interact. Ecotones between forest and grassland, for example, often have higher biodiversity than either adjacent biome because they combine species from both plus unique edge-adapted organisms. These transition zones are also the most sensitive to environmental change, which makes them important indicators but poor candidates for simplistic categorization. Something worth noting is that the concept of a closed biosphere applies strictly to Earth only in a theoretical sense. Matter does enter and leave the atmosphere through meteorite deposition and atmospheric escape, but these fluxes are negligible compared to internal cycling. The real boundary that matters is energetic. Earth receives a constant input of solar radiation and radiates heat back into space. The biosphere is the mechanism that captures a fraction of that incoming energy and routes it through living systems before it degrades to heat. Without that continuous energy flow, the cycling stops and the system freezes into chemical equilibrium. Decomposers get far less attention than they deserve in popular explanations. Fungi, bacteria, and detritivorous invertebrates break down organic matter and release nutrients back into the soil and water. Without them, carbon, nitrogen, phosphorus, and every other essential element would remain locked in dead tissue. A single gram of healthy forest soil can contain billions of bacteria and millions of fungal spores. The total biomass of soil microbes on Earth exceeds that of all plant and animal biomass combined. They're the invisible infrastructure that makes everything else possible.