Why Most People Misunderstand How the Biosphere Actually Works
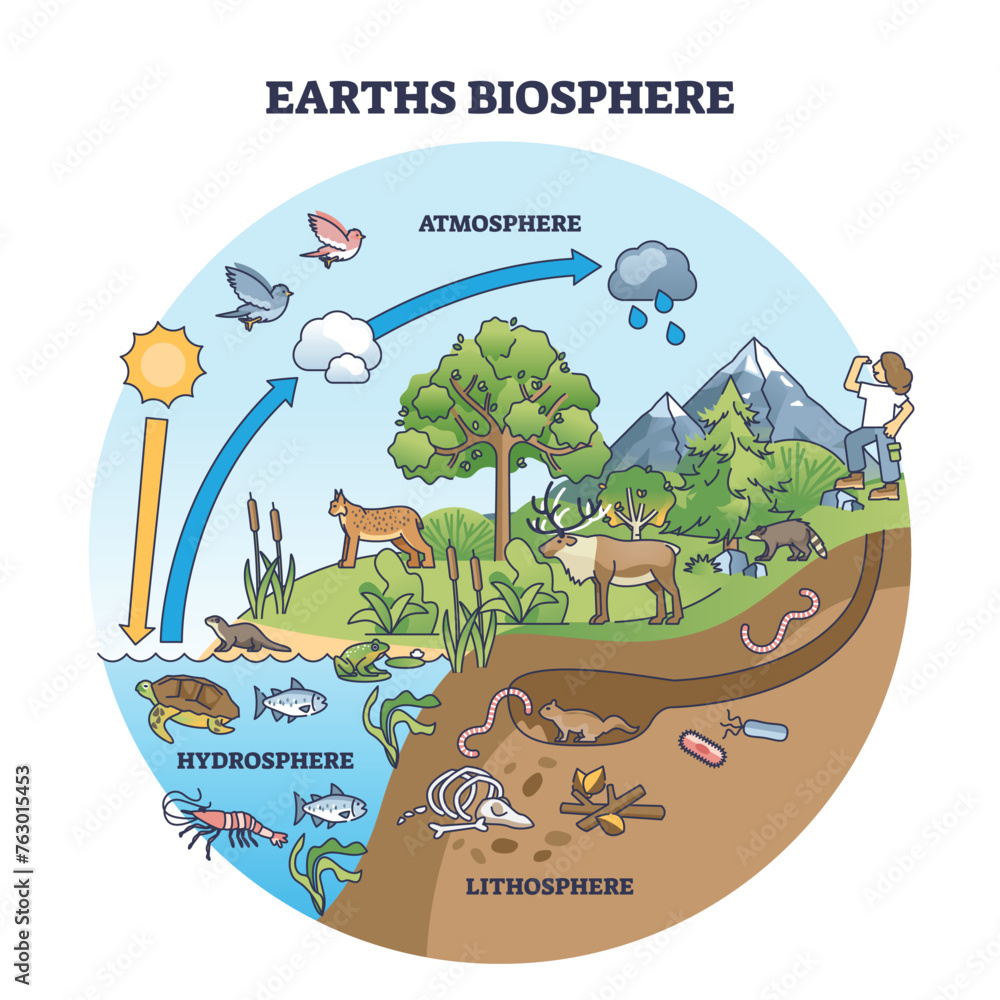
Most people treat the biosphere like a collection of ecosystems sitting side by side. That's not how it functions. The biosphere is a single continuous thermodynamic system where energy flows from sunlight through multiple trophic levels, and matter cycles endlessly between organisms and their physical environment. Carbon, nitrogen, phosphorus — none of these stay in one place. They move through soil, water, atmosphere, and living tissue in ways that are harder to track than most textbooks admit.The Biosphere A Complex And Underappreciated Natural System
I spent years modeling biogeochemical cycles for a watershed management group, and the first thing we had to unlearn was the assumption that boundaries matter much. A forest upstream affects water chemistry thirty kilometers downstream. Microbes in a peat bog emit methane that enters the same atmospheric pool as emissions from a feedlot two hundred miles away. The biosphere doesn't care about your map lines. The core mechanism is simpler than it appears and more fragile at the same time. Solar energy enters, drives photosynthesis, and gets passed along food webs. At every transfer, roughly ninety percent of that energy is lost as heat. That's why ecosystems have limited trophic levels. Most only support three or four before there's not enough energy left to sustain another consumer tier. The remaining ten percent fuels biomass production, respiration, and decomposition. Decomposition is where things get complicated and where beginners consistently underestimate feedback loops. Microbial decomposers don't just break things down passively. Their activity rate depends on temperature, moisture, substrate quality, and the presence of competing organisms. I've seen models fail because someone assumed decomposition was a fixed function of mass. It isn't. In a temperate forest floor, leaf litter might take eight to fourteen months to fully decompose depending on fungal community composition and seasonal rain patterns. In a tropical rainforest, the same mass breaks down in six to nine weeks. Get that difference wrong in a carbon budget calculation and your numbers are off by a factor of three or four within a single growing season.
How to actually measure biosphere dynamics without going crazy
Start with flux measurements rather than stock measurements. Standing biomass tells you less than the rate at which carbon enters or leaves a system. Eddy covariance towers measure net ecosystem exchange directly. They're expensive but they give you real-time data on whether a landscape is a source or a sink. I've used flux data from two sites in the Pacific Northwest — one old-growth conifer stand, one recently clear-cut second growth — and the difference in annual carbon uptake was roughly 4.2 tonnes per hectare per year. That's not theoretical. That's what the instruments recorded over a twelve-month period. For nutrient cycling, isotope tracing is the most reliable method I've worked with. Stable isotopes of nitrogen (15N) and carbon (13C) let you track where atoms actually go rather than assuming they stay put. You apply a small pulse of enriched material and monitor its movement through soil, plant tissue, and microbial biomass over time. It's precise. It's also labor-intensive and requires mass spectrometry access, which means budget and timeline considerations that most student projects ignore until it's too late. Remote sensing fills gaps but introduces its own errors. NDVI and related vegetation indices correlate well with gross primary production in dense canopies. They break down in sparse or heterogeneous landscapes. I once reviewed a satellite-based biomass estimate for a mixed shrub-steppe transition zone that overestimated actual carbon storage by roughly sixty percent. The sensors couldn't distinguish between live woody shrub cover and dead standing material. Ground truthing would have caught that in a single field visit.
The parts nobody talks about
The subsurface biosphere is massive and mostly ignored in introductory courses. Microbial biomass in soil below the root zone, in deep aquifers, in continental crust fractures — recent estimates suggest this hidden compartment may contain as much carbon as all aboveground vegetation combined. These organisms grow incredibly slowly. Some divide once every few hundred to thousand years. They're metabolically active but at rates so low they barely register in standard respiration measurements. When you drill into these zones or perturb them through fracking or deep geothermal projects, you're releasing ancient carbon stores into active cycles that the atmosphere isn't prepared to absorb quickly without consequences. Another overlooked factor is the role of mycorrhizal networks in connecting plant communities. These fungal symbionts transfer carbon, nitrogen, and phosphorus between individual plants, sometimes across species boundaries. The classic "wood wide web" framing is oversimplified and occasionally misleading, but the underlying phenomenon is real and measurable. I've pulled soil cores where phosphorus labeled with 32P appeared in neighboring plant tissue within seventy-two hours, moved through hyphal pathways rather than through soil solution diffusion. This changes how you think about nutrient limitation. Plants in nutrient-poor soils aren't always starving — they're being fed by neighbors through a network that standard soil tests completely miss.
Get the Full Details
Where the standard approaches fail
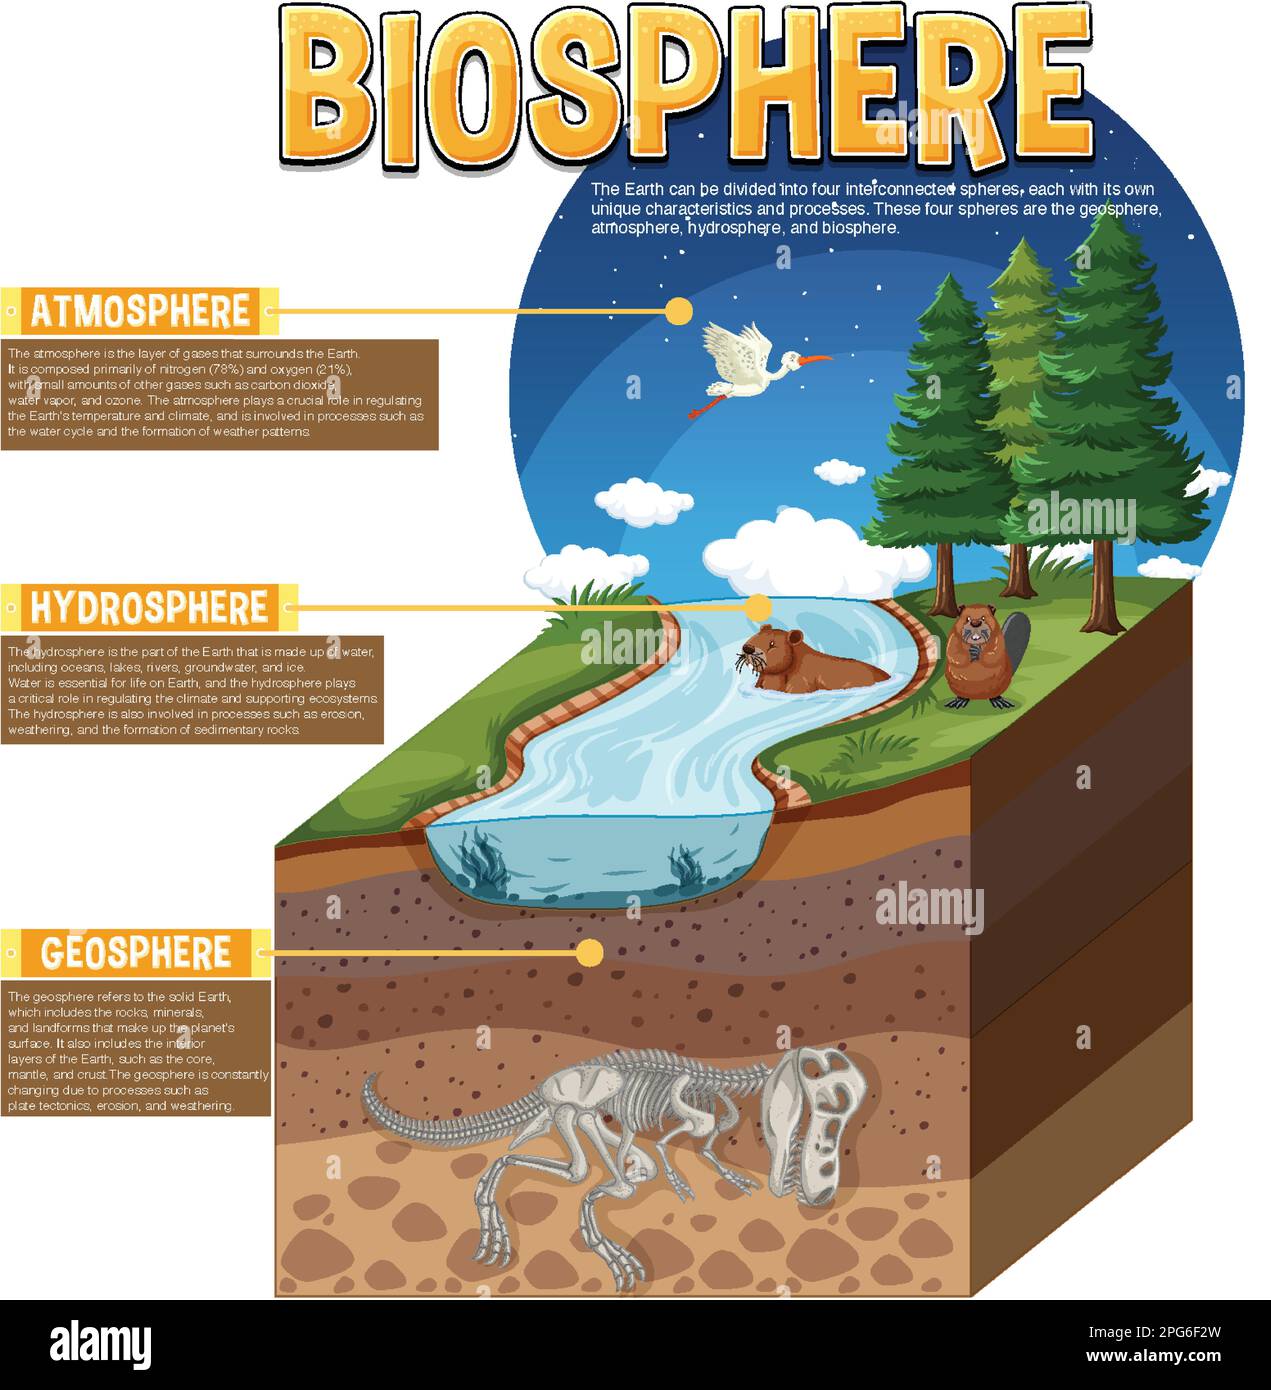
Compartment models are the industry standard for representing biosphere dynamics. You define pools — atmosphere, vegetation, soil organic matter, dissolved organic carbon — and fluxes between them. They're intuitive and computationally tractable. They're also frequently wrong in ways that compound over time. The problem is that real biosphere processes are nonlinear and context-dependent. A temperature increase that speeds decomposition in one biome might inhibit it in another by altering microbial community composition. A drought that reduces photosynthesis in a grassland might increase it in a shrubland by reducing competition for water. Parameter uncertainty is the real killer. Most biosphere models use literature-derived constants for decomposition rates, respiration Q10 values, and nutrient use efficiencies. These constants come from controlled experiments conducted under idealized conditions. Real ecosystems don't match those conditions. When I recalibrated a Terrestrial Biosphere Model for a specific boreal site, the default parameters produced a spring carbon uptake curve that peaked three weeks too early and underestimated summer respiration by about thirty-five percent. Switching to site-specific parameter values derived from local flux data brought the simulation into alignment. The model structure itself was fine. The inputs were generic. Another common failure mode is ignoring disturbance regimes. Fire, pest outbreaks, windthrow, logging — these events reset successional clocks and redistribute carbon and nutrients rapidly. Most models treat disturbance as a stochastic perturbation rather than a structured ecological driver. In boreal forests, fire return intervals of eighty to one hundred fifty years are the norm. A model that doesn't account for this will systematically overestimate long-term carbon storage because it assumes steady-state accumulation that never actually occurs.
Practical workaround for field constraints
When you can't afford eddy covariance towers or isotope facilities, there's a middle-ground approach that works reasonably well. Combine high-frequency soil respiration measurements with weekly biomass sampling and monthly soil nutrient extraction. Use species-specific allometric equations to estimate aboveground carbon stocks from diameter measurements. Cross-validate with whatever satellite data is available for your region. It won't match the precision of dedicated flux sites, but for a lot of management-level questions — is this landscape gaining or losing carbon? Are nutrient cycles accelerating or slowing? — it gives you answers within twenty to thirty percent accuracy, which is usually sufficient for decision-making. The key is consistency. Measuring the same variables at the same intervals across multiple seasons and years lets you detect trends even if individual measurements have error. I've seen too many one-off surveys where someone measures soil carbon in September and calls it a year. Soil respiration and microbial activity peak in late summer in most temperate systems. A single September sample will overestimate annual carbon input if you're inferring flux from standing stocks. Run measurements across at least two full growing seasons before drawing conclusions. There's no clean endpoint to understanding the biosphere. It's too large, too interconnected, and too responsive to small changes for any single model or dataset to capture it fully. The best you can do is improve your measurements, acknowledge where your assumptions are weakest, and keep updating your understanding as new data becomes available. The system keeps changing whether you're watching or not.