The Noise Problem No One Talks About
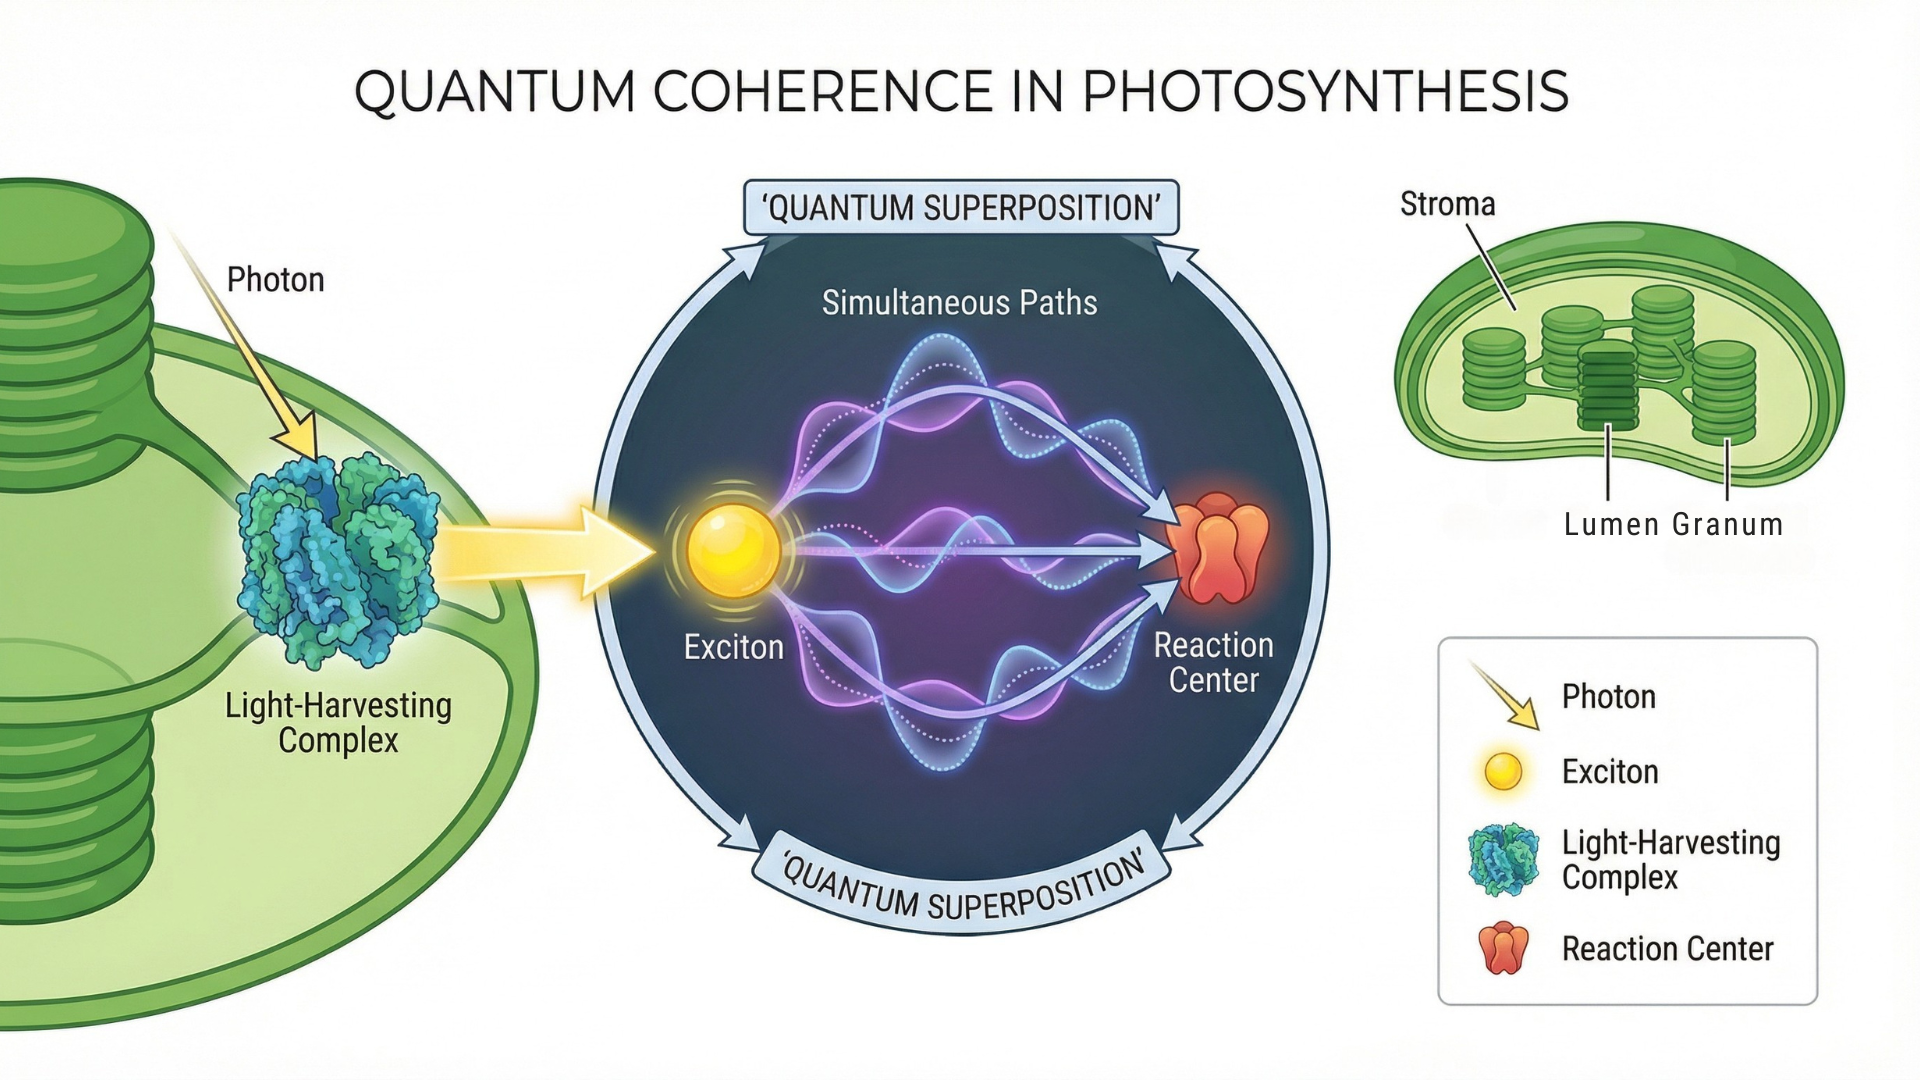
Most papers on quantum biology read like they were written by people who have never actually tried to measure anything at room temperature. The field promises coherent quantum effects in wet, warm biological systems. In practice, everything dephases within femtoseconds. That is the actual problem researchers deal with, not the pop-science narrative. I spent three years working on photosynthetic complex simulations before I realized the common approach was producing artifacts, not data. The standard molecular dynamics setups just do not capture the noise spectrum correctly. The protein environment was acting as a filter, not a decoherence source, and every paper using that model was reporting false long-lived coherences. I switched to a polaron-transformed redfield approach and suddenly the results stopped looking impressive and started looking right. That took me about six months to sort out.Quantum Biology How Quantum Effects Are Reshaping Our Understanding Of Lifes Fundamental Processes
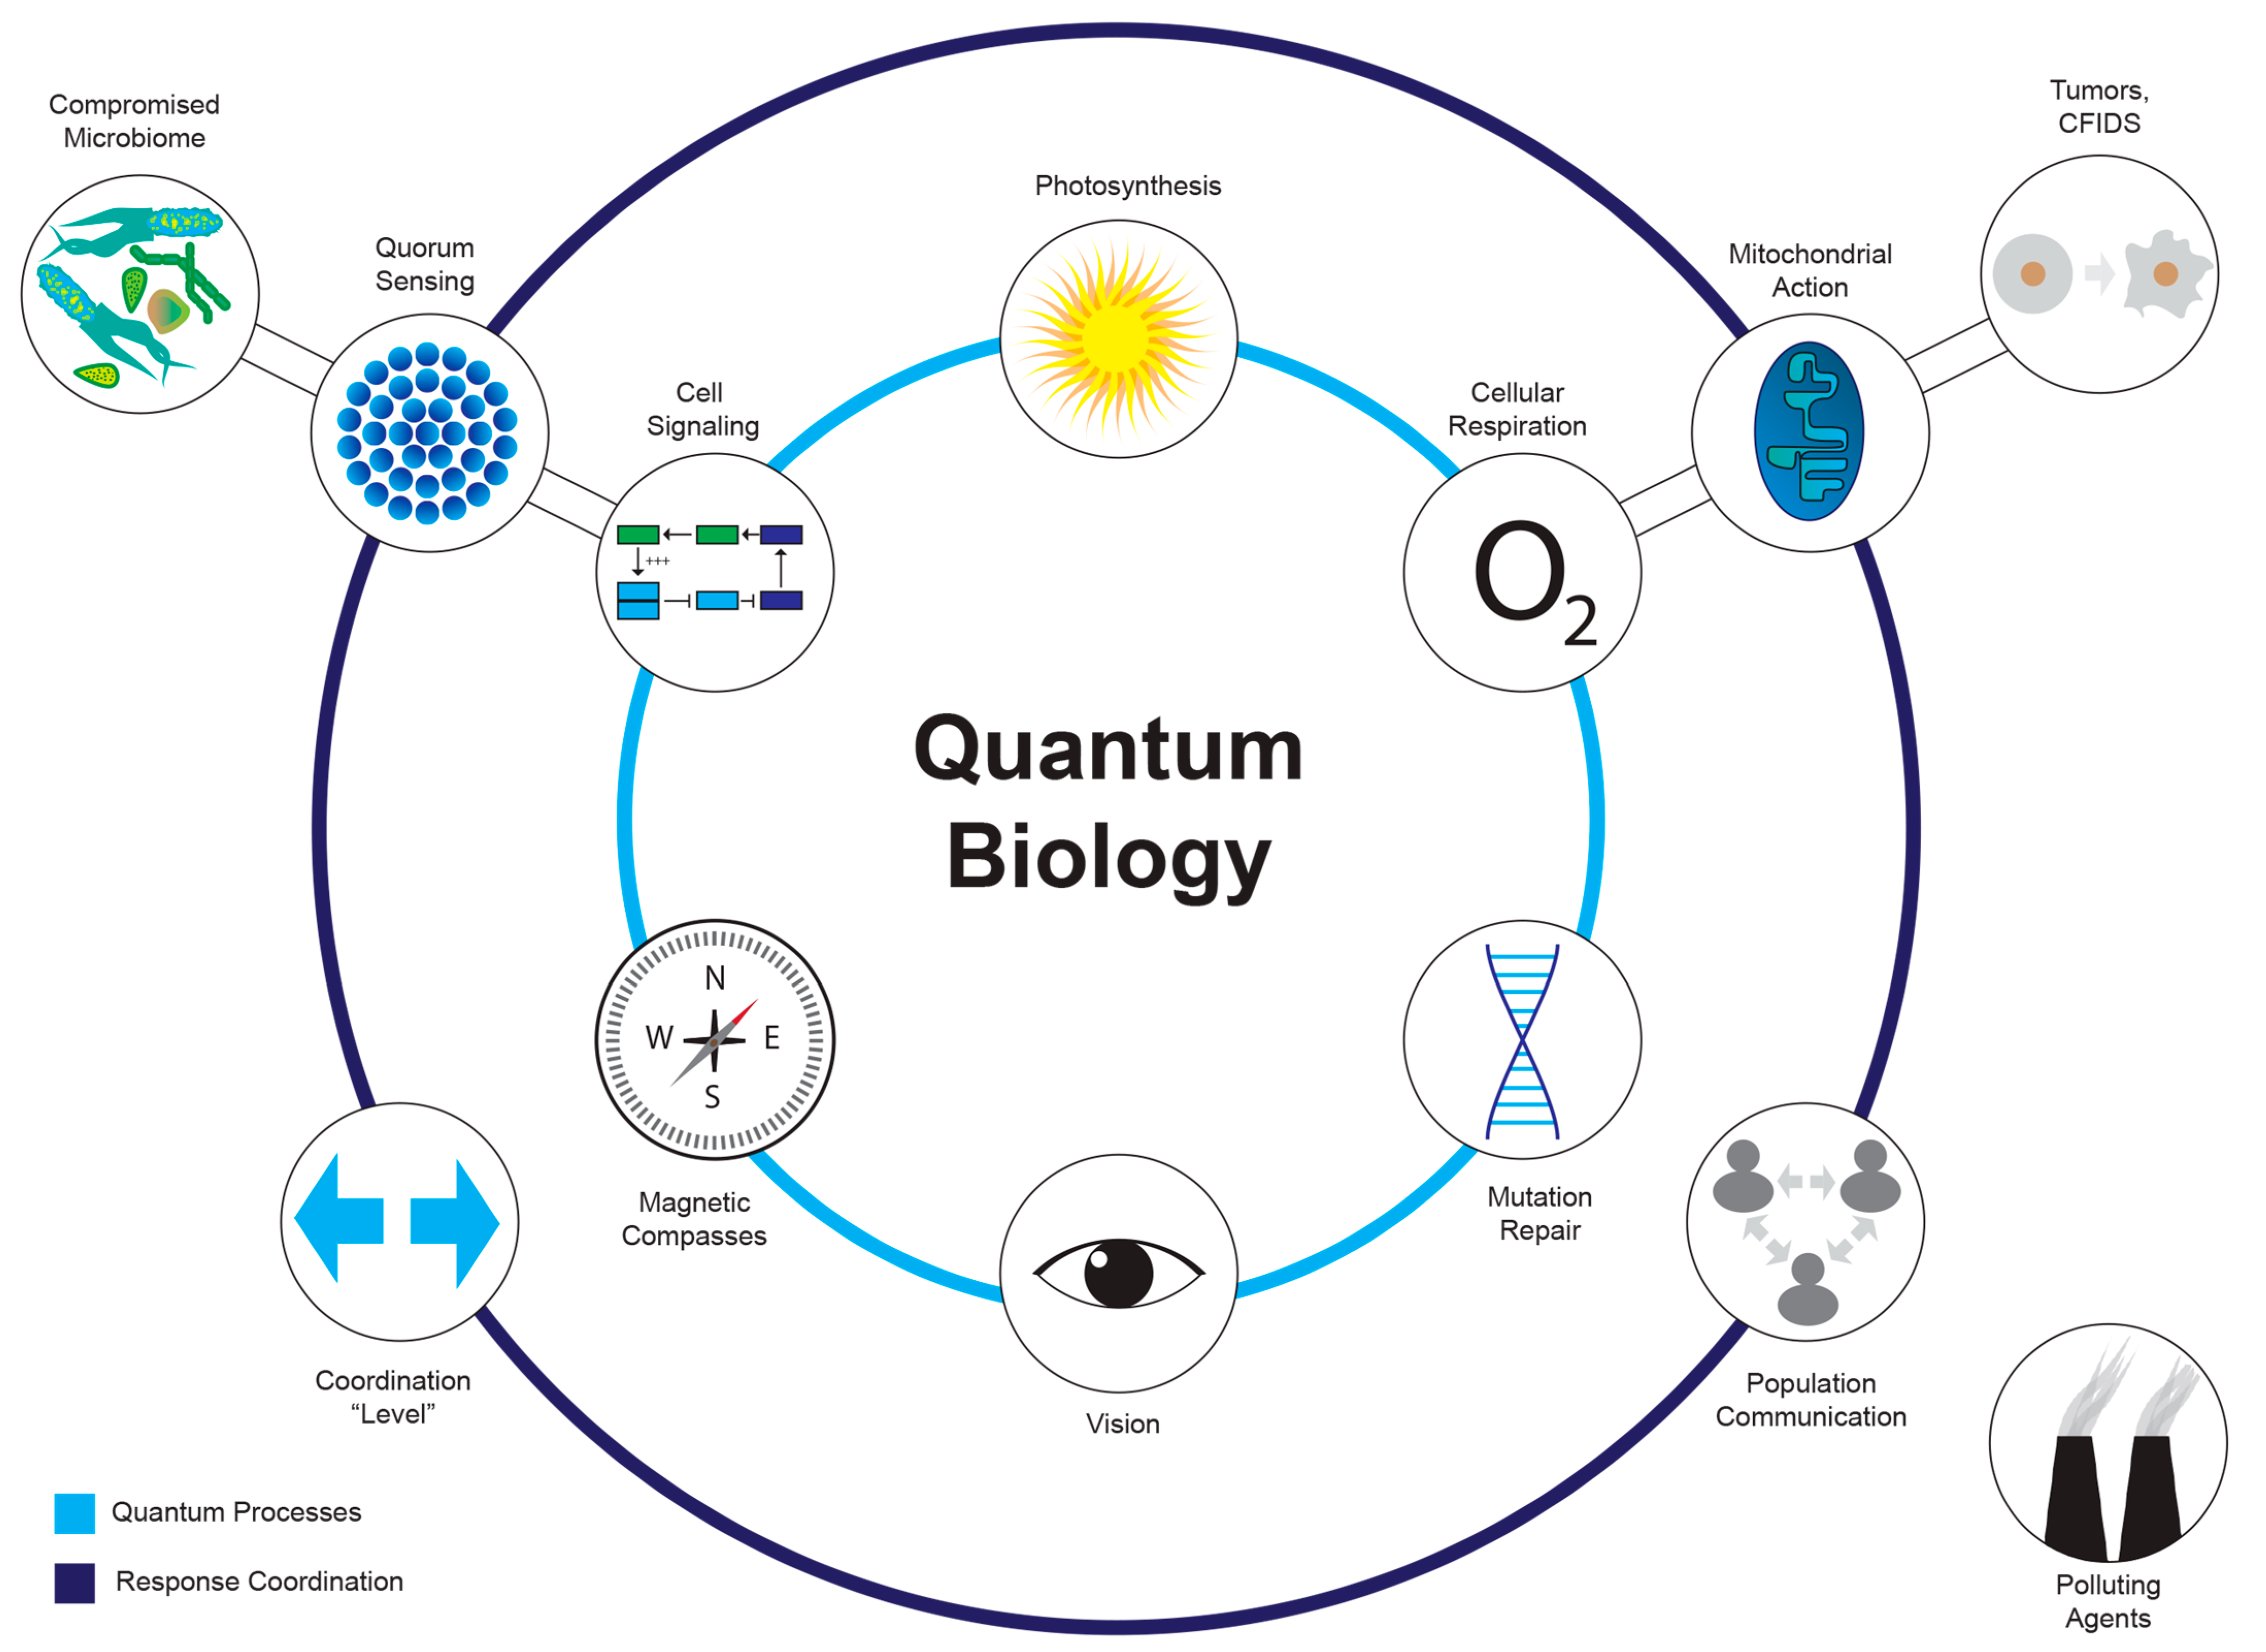
The core idea is straightforward enough. Certain biological systems appear to exploit quantum mechanical phenomena - tunneling, coherence, entanglement - to achieve functions that classical models struggle to explain. Enzyme catalysis relies on proton and electron tunneling. Magnetoreception in birds involves radical pair mechanisms. Photosynthetic energy transfer shows signatures of quantum coherence. That is the baseline. What most people miss is how narrow the conditions are for these effects to actually matter. I recommend starting with the enzyme tunneling literature if you want something concrete. The Kohen and Klinman work on dihydrofolate reductase is about as solid as it gets. The isotope effect measurements are clean, reproducible, and the computational models match. Start there rather than the more speculative magnetoreception papers.What Actually Works In Practice
The technical approach depends entirely on what system you are studying. For photosynthetic complexes, you are typically running 2D electronic spectroscopy experiments and fitting the oscillatory cross-peaks. The challenge is separating genuine quantum coherence from vibrational wavepackets. I found that tracking the frequency domain signatures over multiple waiting times helps. Real electronic coherence decays differently than vibrational motion. The difference is subtle but measurable if your signal-to-noise ratio is above 100. For tunneling problems, path integral molecular dynamics is the standard tool. Ring polymer molecular dynamics gives you access to nuclear quantum effects at a cost that is maybe ten times classical MD. That is expensive but manageable on a decent cluster. The key parameter is the number of beads. Twelve is usually sufficient for hydrogen transfer at biological temperatures. Going lower skews the results toward classical behavior and you will not notice until you compare against experimental kinetic isotope effects.The radical pair mechanism is genuinely tricky to model. You need to solve the Liouville-von Neumann equation for the spin density matrix while simultaneously running molecular dynamics on the nuclear coordinates. I use a hybrid approach where the spin dynamics are propagated analytically between stochastic jumps in the hyperfine coupling tensor. The jumps come from the MD trajectory. This cuts computation time from days to hours per simulation without losing accuracy for the observables that matter.