Specialization Works Until It Doesn't
Narrow niches look elegant on paper. A specialist occupies a very specific set of environmental conditions and resource types, and this lets them outcompete generalists within that narrow band. You see the pattern everywhere: the koala eating only eucalyptus leaves, the actinia sea anemone glued to a single wave-wash zone on rocky shores, the fig wasp that can only pollinate one fig species. Specialization is an efficiency strategy. It reduces competition by carving out a slice of the environment so small that most other organisms cannot access it at all. The trade-off is brutal and immediate. When the niche shifts, even slightly, the specialist has nowhere to go. Generalists shuffle between resources. Specialists are locked in.
Precision Meets Survival How Biological Niche Specialization Defines Lifes Tightrope In The Living World
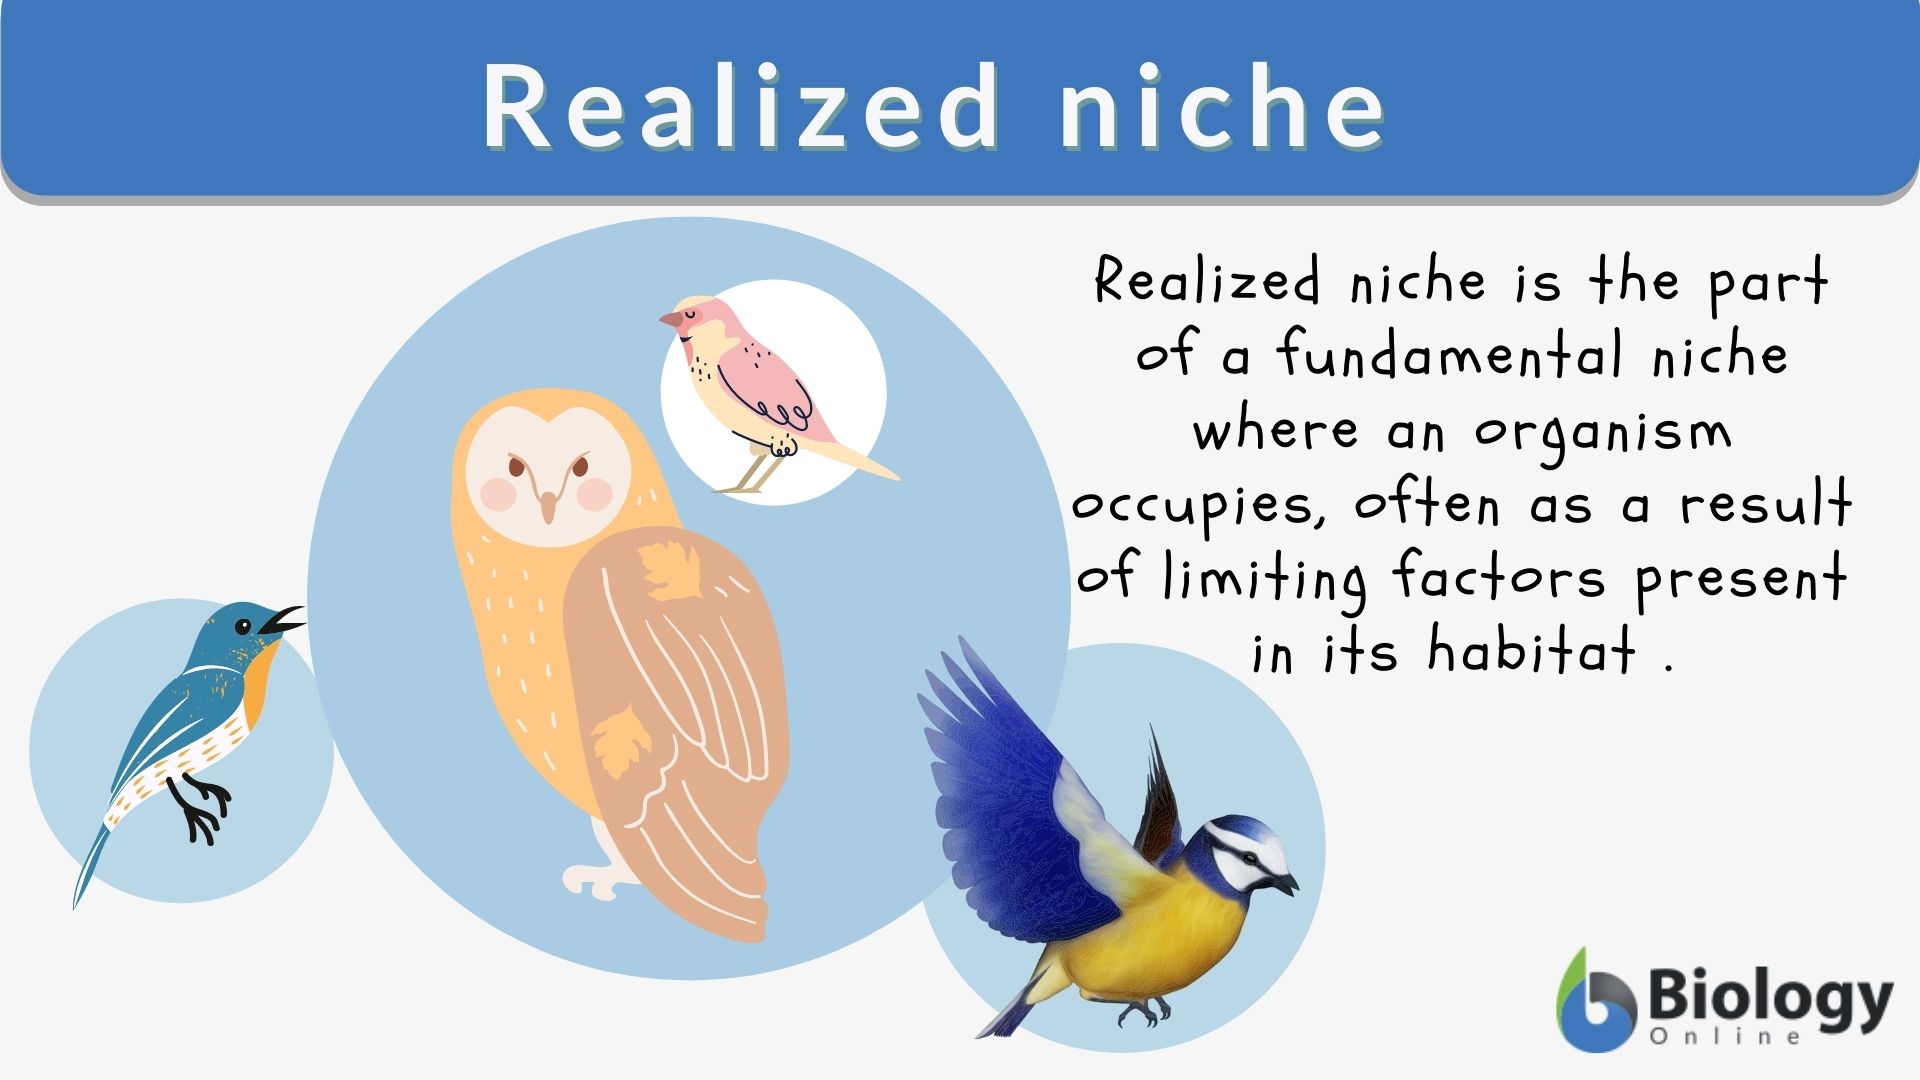
The tightrope framing comes from the fact that specialists live in a narrow envelope of tolerance. This is not a poetic observation. It is measurable. Hutchinsonian niche theory defines the fundamental niche as the full range of abiotic conditions an organism can tolerate, and the realized niche as the subset it actually occupies once biotic interactions are factored in. For a specialist, both values collapse toward a single point. A change of a few degrees in water temperature, a one percent shift in soil pH, or the introduction of a single competitor can wipe the realized niche down to zero. I spent three field seasons studying a population of stream-breeding salamanders in the southern Appalachians. These were Plethodon jordani, lungless foresters that rely on a very specific moisture window and a specific range of leaf litter depth for egg deposition. We mapped their microhabitat use across four watershed segments and found something that standard niche models did not predict. The apparent population stability in two of those segments was masking a steep narrowing of the realized niche. The salamanders were persisting, yes, but only because a previously rare predator, a larval dragonfly, had colonized those streams five years earlier. The salamanders were surviving through behavioral avoidance alone. They were occupying habitat that had become marginal, and the demographic data suggested this was unsustainable beyond another two to three generations. My workaround involved switching from presence-only surveys to a mark-recapture model that included microhabitat covariates measured at the individual level, rather than at the plot level. Plot-level data smoothed over the micro-variation that actually determined survival. At the individual scale, we found that survival dropped off sharply once leaf litter depth fell below 3.2 centimeters. Below that threshold, egg desiccation rates spiked and predation exposure increased because the animals could no longer retreat into the litter matrix. That 3.2 centimeter value became our early warning indicator. It was also a value that would never show up in a coarse-scale niche model.
Why Specialists Lose Less Than They Appear To
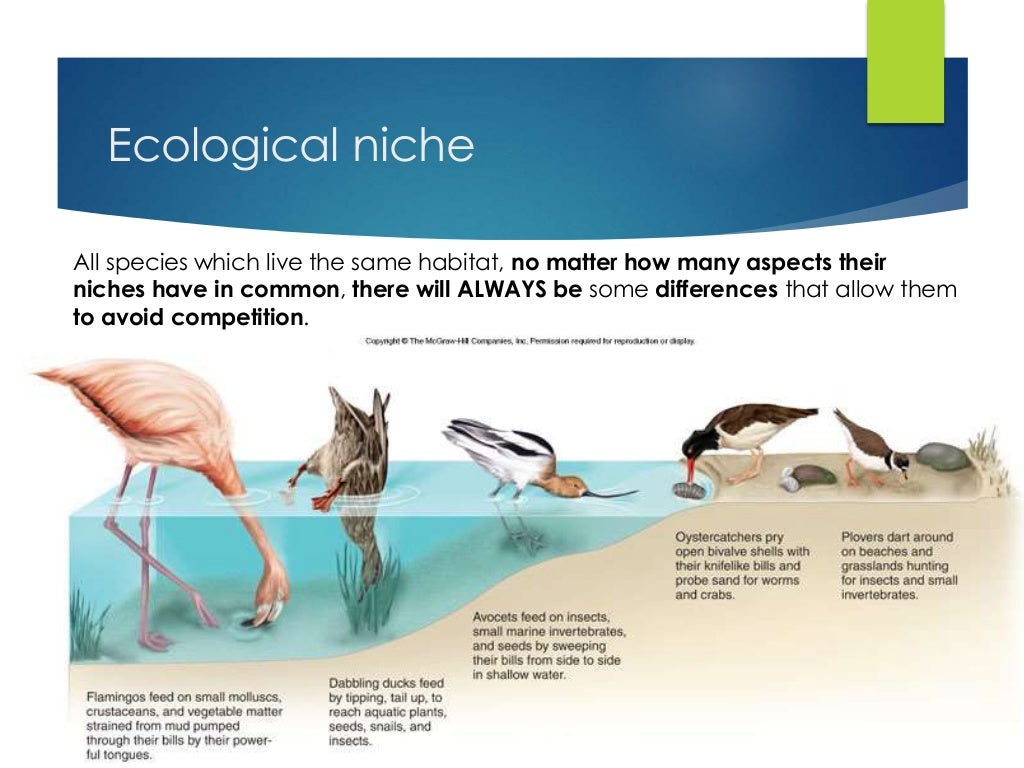
The conventional narrative treats specialists as fragile by default. That is partly correct but it misses a structural reason why specialists persist at all. Specialization is not merely the absence of options. It is the product of competitive exclusion working over long time scales. In stable environments, generalists spread their effort thin across many resources, which means each resource receives less individual attention and lower exploitation efficiency. Specialists concentrate their physiological and behavioral machinery on one resource type and achieve higher competitive dominance within that slice. This is niche partitioning in action, and it is why specialist coexistence is possible in diverse communities. Each species occupies its own sliver, and the community as a whole utilizes the full resource spectrum without direct overlap. The counter-intuitive part is that this partitioning creates vulnerability. When environmental conditions shift along a single axis, every specialist in the system shifts in the same direction at the same time. There is no asynchrony. Generalist populations, by contrast, contain internally asynchronous sub-populations using different resources, which provides a built-in buffer. This is why specialist-dominated systems can appear stable for decades and then collapse rapidly during regime shifts. The stability you observe is not resilience. It is precarious equilibrium. Another common misunderstanding involves the relationship between geographic range size and specialization. Many ecologists assume specialists always have small ranges, but this is not a necessary condition. A specialist can have a very large range if its narrow niche requirement happens to be abundant across a broad area. The emperor penguin is a dietary specialist feeding almost exclusively on Antarctic krill and fish, yet its range spans thousands of kilometers of coast. Range size and niche breadth are correlated but not coupled. Confusing the two leads to flawed extinction risk assessments in conservation planning.
Get the Full Details

Practical Implications For Monitoring And Management
If you are working in habitat assessment, species distribution modeling, or conservation planning, there are a few things that will trip you up if you treat specialists like generalists with narrow preferences. First, occurrence data alone is insufficient for specialists. A single presence record tells you very little about whether the site is core habitat or marginal habitat. Marginal sites support low survival and function as ecological traps. Without demography, you cannot distinguish the two. I have seen management plans built entirely on occurrence data from eBird and iNaturalist, which produces maps that look comprehensive but contain large swaths of unusable habitat. For a specialist, those unusable patches are the majority of the map. Second, occupancy modeling with detection probability corrections helps, but it still does not capture microhabitat dependency. The salamander example above illustrates this clearly. The species was detected across its full historic range, but detection does not equal viability. When we layered in microhabitat measurements, the viable area shrank by roughly forty percent. That number changed the entire management recommendation for two of the watershed segments.
Third, climate niche projections for specialists tend to overestimate future range loss because they assume niche conservatism, which is usually reasonable, but they also assume that the organism can track its niche through dispersal. Most specialists cannot. Their dispersal ability is often limited precisely because their morphology and behavior are optimized for their narrow niche. A seed that is perfectly adapted for gravity dispersal into leaf litter cannot colonize a new mountain slope fifty kilometers away when the climate shifts. This dispersal limitation is a first-order constraint, not a secondary detail. Fourth, the concept of niche tracking is useful but easily misapplied. In practice, specialists track their niche through microrefugia, not macro-range shifts. A shaded north-facing slope, a seeps, a canopy gap, or a cold-air drainage zone can maintain the required conditions while the surrounding landscape shifts out of tolerance. These microrefugia are typically small, fragmented, and rarely represented in coarse-resolution habitat models. If your model resolution is above one hundred meters, you are unlikely to resolve them.
Where Specialization Fails Completely
There are scenarios where the specialization framework breaks down as a predictive tool. Rapid anthropogenic change is the primary example. The niche concept assumes a relatively stable environmental baseline, which is increasingly absent from most terrestrial and aquatic systems. When change velocity exceeds the generation time of the organism, niche-based predictions become unreliable within a single decade. The model assumes equilibrium. The system is in nonequilibrium. A second failure mode occurs with omnivory and dietary switching that appears to contradict specialization. Some species labeled as specialists will shift to alternative resources under acute stress. This is not evidence that the original classification was wrong. It is evidence that the specialist status describes the normal operational state, not a hard physiological limit. However, this flexibility is usually costly. Switching resources requires altered foraging behavior, increased energy expenditure, and exposure to novel predators or competitors. The demographic cost of switching is often high enough that populations relying on it decline even while they technically persist. A third limitation is that specialization is trait-specific, not organism-wide. An organism can be a specialist in one dimension and a generalist in another. A bird might feed on a single insect species while nesting in a wide variety of tree cavities. Conservation assessments that aggregate niche breadth across all dimensions will misrepresent the actual constraint. The feeding niche is the bottleneck, not the nesting niche. Treating the species as a moderate generalist because of nesting flexibility will produce a management plan that fails to protect the insect prey.

Finally, specialist-generalist continua are frequently collapsed into binary categories in policy documents. They are not binary. Niche breadth exists on a continuum, and the relevant axis depends entirely on the ecological question being asked. A herbivorous insect may be a specialist at the plant genus level but a generalist at the family level. Both statements are true. The management implication changes depending on which taxonomic resolution matters for the resource being protected.
What Actually Works In Practice
If you need to assess specialist populations or design protection strategies around them, the approach that has worked consistently in my experience combines three elements: fine-scale microhabitat mapping, demographic monitoring, and climate envelope modeling run at resolution fine enough to resolve microrefugia. Microhabitat mapping should operate at the scale of the individual organism, not the plot or the landscape unit. In the salamander project, we used handheld laser rangefinders and soil probes to measure litter depth, moisture content, and substrate temperature at ten-centimeter intervals along transects. This took more time than standard quadrat-based surveys, but it produced data that actually predicted survival. Standard quadrats at two-meter intervals missed the critical variation entirely. Demographic monitoring requires marking individuals and returning to re-estimate survival and reproduction over multiple seasons. Occurrence surveys can be done in a single pass. Survival estimates cannot. The difference in information content between the two approaches is the difference between knowing a population exists and knowing whether it is growing, stable, or declining. For a specialist, that distinction is the entire management question.
Climate envelope modeling for specialists should incorporate downscaled projections and microrefugium identification, not just bioclimatic variables. WorldClim at one-kilometer resolution will miss the thermal and moisture gradients that specialists actually respond to. I have used terrain-based microclimate modeling derived from LiDAR canopy cover data and digital elevation models at ten-meter resolution, which captures shade patterns and cold-air pooling well enough to identify likely refugia. The output is still an approximation, but it is an approximation grounded in physical reality rather than interpolated climate averages. There is no shortcut around this level of effort for specialists. Generalists tolerate coarse data because their responses are buffered across multiple resources and habitats. Specialists do not. The precision of the niche demands the precision of the assessment. Anything less produces confident but incorrect conclusions, which is worse than no conclusions at all.