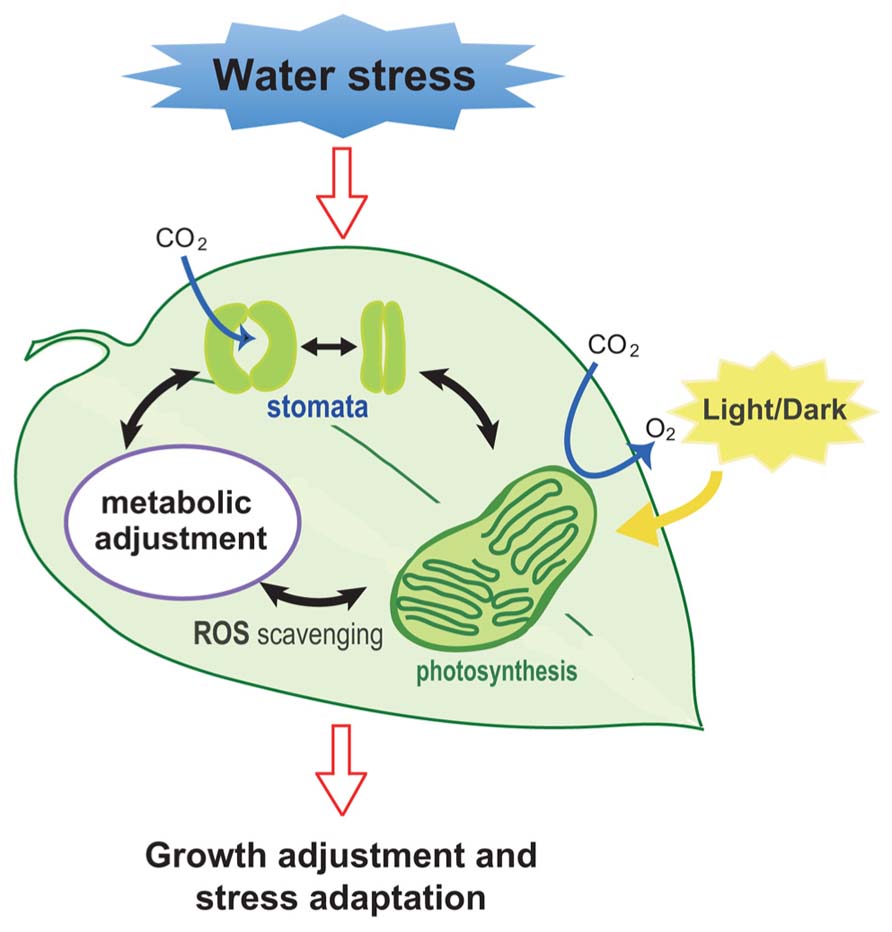
Understanding Plasmolysis in Plant Cell Water Regulation
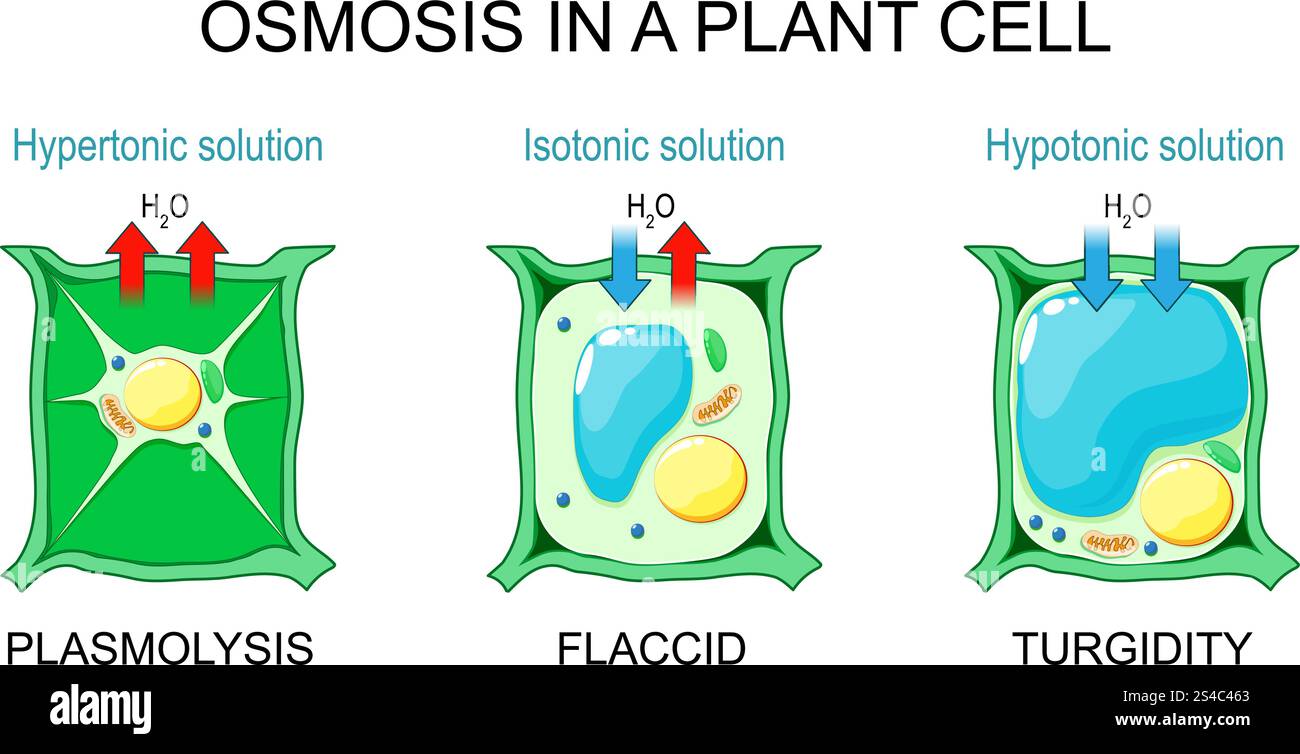
Plant cells have a rigid cell wall surrounding a flexible plasma membrane, and when water moves out of the cell faster than it can be replaced, the membrane detaches from that wall. This separation is plasmolysis, and it happens whenever the external solution has a lower water potential than the cell's cytoplasm. I spent a lot of time studying this under a microscope in undergrad labs, but seeing it happen in real tissue samples during drought conditions gave me a much clearer picture of what the textbook diagrams were actually trying to show. When a plant cell is placed in a hypertonic environment, water exits through the semi-permeable plasma membrane by osmosis. The central vacuole shrinks first since it holds most of the cell's water content, and as turgor pressure drops toward zero, the protoplast begins to pull inward. Initially you get flaccidity where the cell softens but the membrane stays close to the wall, then complete plasmolysis where clear gaps form between the membrane and the cellulose framework. Xerophytic plants like cacti and sagebrush handle this quite differently from mesophytes like lettuce or Arabidopsis. Their cells accumulate compatible solutes such as proline, glycine betaine, and soluble sugars to lower internal water potential without disrupting enzyme function. This osmotic adjustment means the cell can continue drawing water from increasingly dry soil rather than immediately entering plasmolysis. I ran into a specific problem once while preparing onion epidermis mounts for a teaching lab. I used a 0.8 M sucrose solution to demonstrate plasmolysis, but nearly every student reported seeing almost no separation between the membrane and cell wall after ten minutes. The issue turned out to be that the onion bulbs had been stored in a cold room at around four degrees Celsius for weeks before we used them. Low temperature slows membrane fluidity and reduces aquaporin channel activity, which dramatically delays water efflux even in highly hypertonic solutions. I switched to using garlic cloves stored at room temperature instead, and the plasmolytic shrinkage became visible within three to four minutes under the same sucrose concentration. The workaround was straightforward once I figured it out, but it took two lab sessions and a bunch of confused students to get there.
Aquaporins are integral membrane proteins that form water channels, and their regulation is one of the most important factors in how quickly a cell enters plasmolysis. Phosphorylation of specific aquaporin residues by kinases like SOS2 can close these channels within minutes of salt stress onset, effectively reducing membrane hydraulic conductivity by up to sixty percent. This isn't just a passive consequence of water loss; it's an active defensive response. The plant is deliberately slowing down its own dehydration to buy time for downstream signaling cascades that trigger protective gene expression. Most beginners miss the distinction between irreversible and reversible plasmolysis. If the hypertonic exposure lasts too long or the solute concentration is extreme, the membrane can become permanently damaged. Lipid phase transitions occur, protein complexes dissociate, and even returning the cell to an isotonic or hypotonic medium won't restore normal function. The cell dies. Reversible plasmolysis typically requires recovery within thirty to sixty minutes depending on species and temperature, and the cell regains turgor once water re-enters through reopened aquaporins and restored proton gradient across the membrane. The plasmolysis method itself is useful for determining the osmotic potential of plant tissues. You prepare a series of solutions with known solute potentials, expose tissue samples to each one, and observe under the microscope whether plasmolysis occurs. The solution where fifty percent of cells show initial plasmolysis gives you the approximate osmotic potential of the cell sap. It's a classical technique, and it still works reasonably well, though modern pressure chamber and psychrometer methods are more precise for research applications.
One counter-intuitive point that comes up often: not all water loss in plants involves plasmolysis. Transpiration through stomata pulls water out of mesophyll cells, but the cell wall maintains structural integrity and the overall tissue doesn't undergo the dramatic protoplast shrinkage you see in isolated cells in hypertonic solutions. Plasmolysis is specifically about osmotic water movement across the plasma membrane into an external hypertonic environment, not about the bulk flow of water through the apoplast or symplast during normal transpiration. Students frequently conflate the two. Another thing that isn't obvious: some halophyte species actually thrive in conditions that would plasmolysis a typical crop plant. Salicornia and Spartina maintain extremely low internal water potentials through massive ion accumulation in their vacuoles, often reaching solute potentials below negative two megapascals. Their cells are essentially in a permanent state of what would look like mild plasmolysis under a microscope, but the structural adaptations of the cell wall and membrane prevent catastrophic collapse. The cell wall elasticity and middle lamella composition differ substantially from non-halophytes, providing mechanical resistance against the inward pulling force. The practical limitation of using plasmolysis as an indicator of plant health is that it doesn't distinguish between reversible osmotic stress and actual cellular damage. A leaf wilting from temporary drought and a leaf suffering membrane lipid peroxidation from severe water deficit can look identical externally. You'd need to combine plasmolysis observations with electrolyte leakage assays or chlorophyll fluorescence measurements to get a reliable assessment of cell viability under stress conditions.
Get the Full Details
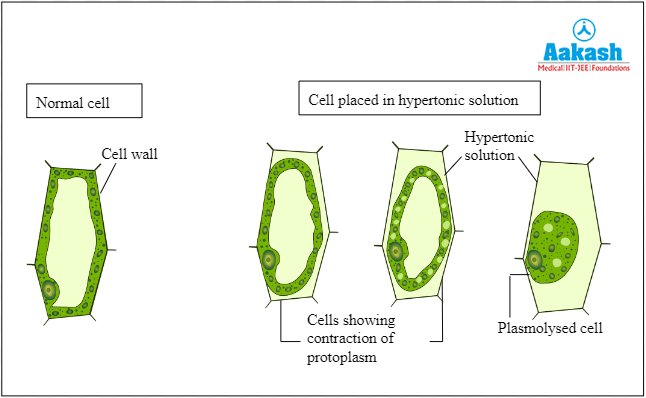
Recovery from plasmolysis depends on several factors including cell wall elasticity, the rate at which water potential equilibrates with the environment, and whether secondary metabolite production has been triggered during the stress period. Some compounds like late embryogenesis abundant proteins and lema genes produce dehydrin proteins that stabilize membranes during desiccation, and their presence or absence can determine whether a cell survives complete plasmolysis and rehydrates successfully or proceeds into programmed cell death.